



-
Livestock, despite being crucial for food security, are responsible for 30% of global anthropogenic methane (CH4) emissions, with 88% originating from enteric fermentation. Among ruminant species, cattle contribute the most (77% of CH4 emissions), followed by buffalo (13%) and other small ruminants (10%)[1]. The global warming potential (GWP) of CH4 is 86 and 28 times higher than carbon dioxide (CO2) over the 20- and 100-year time scales, respectively[2]. CH4 is a potent greenhouse gas that, despite its comparatively low atmospheric concentration, contributes to nearly 30% of global warming. Furthermore, CH4 emissions also diminish the animal productivity by causing a 2%−12% loss of ingested feed energy. Due to high GWP and short atmospheric lifespan, mitigating CH4 emissions presents a significant opportunity to meet the Paris Agreement targets and accelerate global warming mitigation efforts[3]. Over the past several years, numerous CH4-reducing strategies have been explored. Among these, the use of anti-methanogenic feed additives such as 3-Nitrooxypropanol (3NOP), halogenated compounds, nitrates, and essential oils have proven to be the most effective[4−7]. However, the practical applicability of anti-methanogenic feed additives such as bromochloromethane, 2-bromoethane sulfonate, bromoform, and chloroform is limited due to concerns related to human and animal health, rumen adaptation, and environmental regulations[2,8,9]. In this context, 3NOP has emerged as an effective compound to reduce CH4 emissions while maintaining animal production. Its commercial product, Bovaer® has been approved by the European Food Safety Authority (EFSA), and is licensed to be used in more than 70 countries[10,11]. However, in some of the major livestock-producing countries such as China and India, its safety and regulatory status is still under review and is not yet fully authorized. This review offers an in-depth analysis of the mechanisms of action of 3NOP, the factors modulating its efficacy, and its impact on animal production and product quality. It also states the current challenges in its practical application and outlines future research directions aimed at optimizing its use for sustainable livestock production.
-
Archaeal taxa play a central role in enteric CH4 generation; therefore, understanding their taxonomic composition and metabolic pathways is essential for interpreting CH4 mitigation strategies. Rumen archaea account for 0.3%−4% of the rumen microbial population[12]. The classification of methanogenic archaea according to the Genome Taxonomy Database[13,14] is summarized in Fig. 1. The rumen methanogenic community is dominated by the members of the order Methanobacteriales, particularly the genera Methanobrevibacter and Methanosphaera, followed by the members of the order Methanomassiliicoccales. The members of genera Methanomicrobium and Methanosarcina are the least abundant. Methanobrevibacter gottschalkii, Methanobrevibacter ruminantium, Methanosphaera, and two species of the Methanomassiliicoccaceae (rumen cluster C, or RCC) collectively make nearly 90% of the rumen methanogenic community. Among these, Methanobrevibacter alone contributes approximately 74%, while the genus Methanosphaera and Methanomassiliicoccaceae together represent the remaining 16%. The composition of rumen archaea may vary with host species, diet, and environmental conditions; however, dominant methanogens appear to be relatively similar across the ruminant species and dietary conditions[13,15,16]. Most Methanobacteriales primarily produce CH4 by reducing CO2 with hydrogen (H2), though some utilize formate, carbon monoxide, or secondary alcohols[17]. Methanosphaera uniquely reduces methanol with H2[18]. Members of the order Methanomassiliicoccales perform methanogenesis using methylated compounds[19], whereas Methanomicrobiales utilize CO2 with H2, formate, and secondary alcohols[17]. In comparison, Methanosarcina exhibits metabolic flexibility, producing CH4 from multiple substrates, including methylated compounds, acetate, H2, and CO2[20].
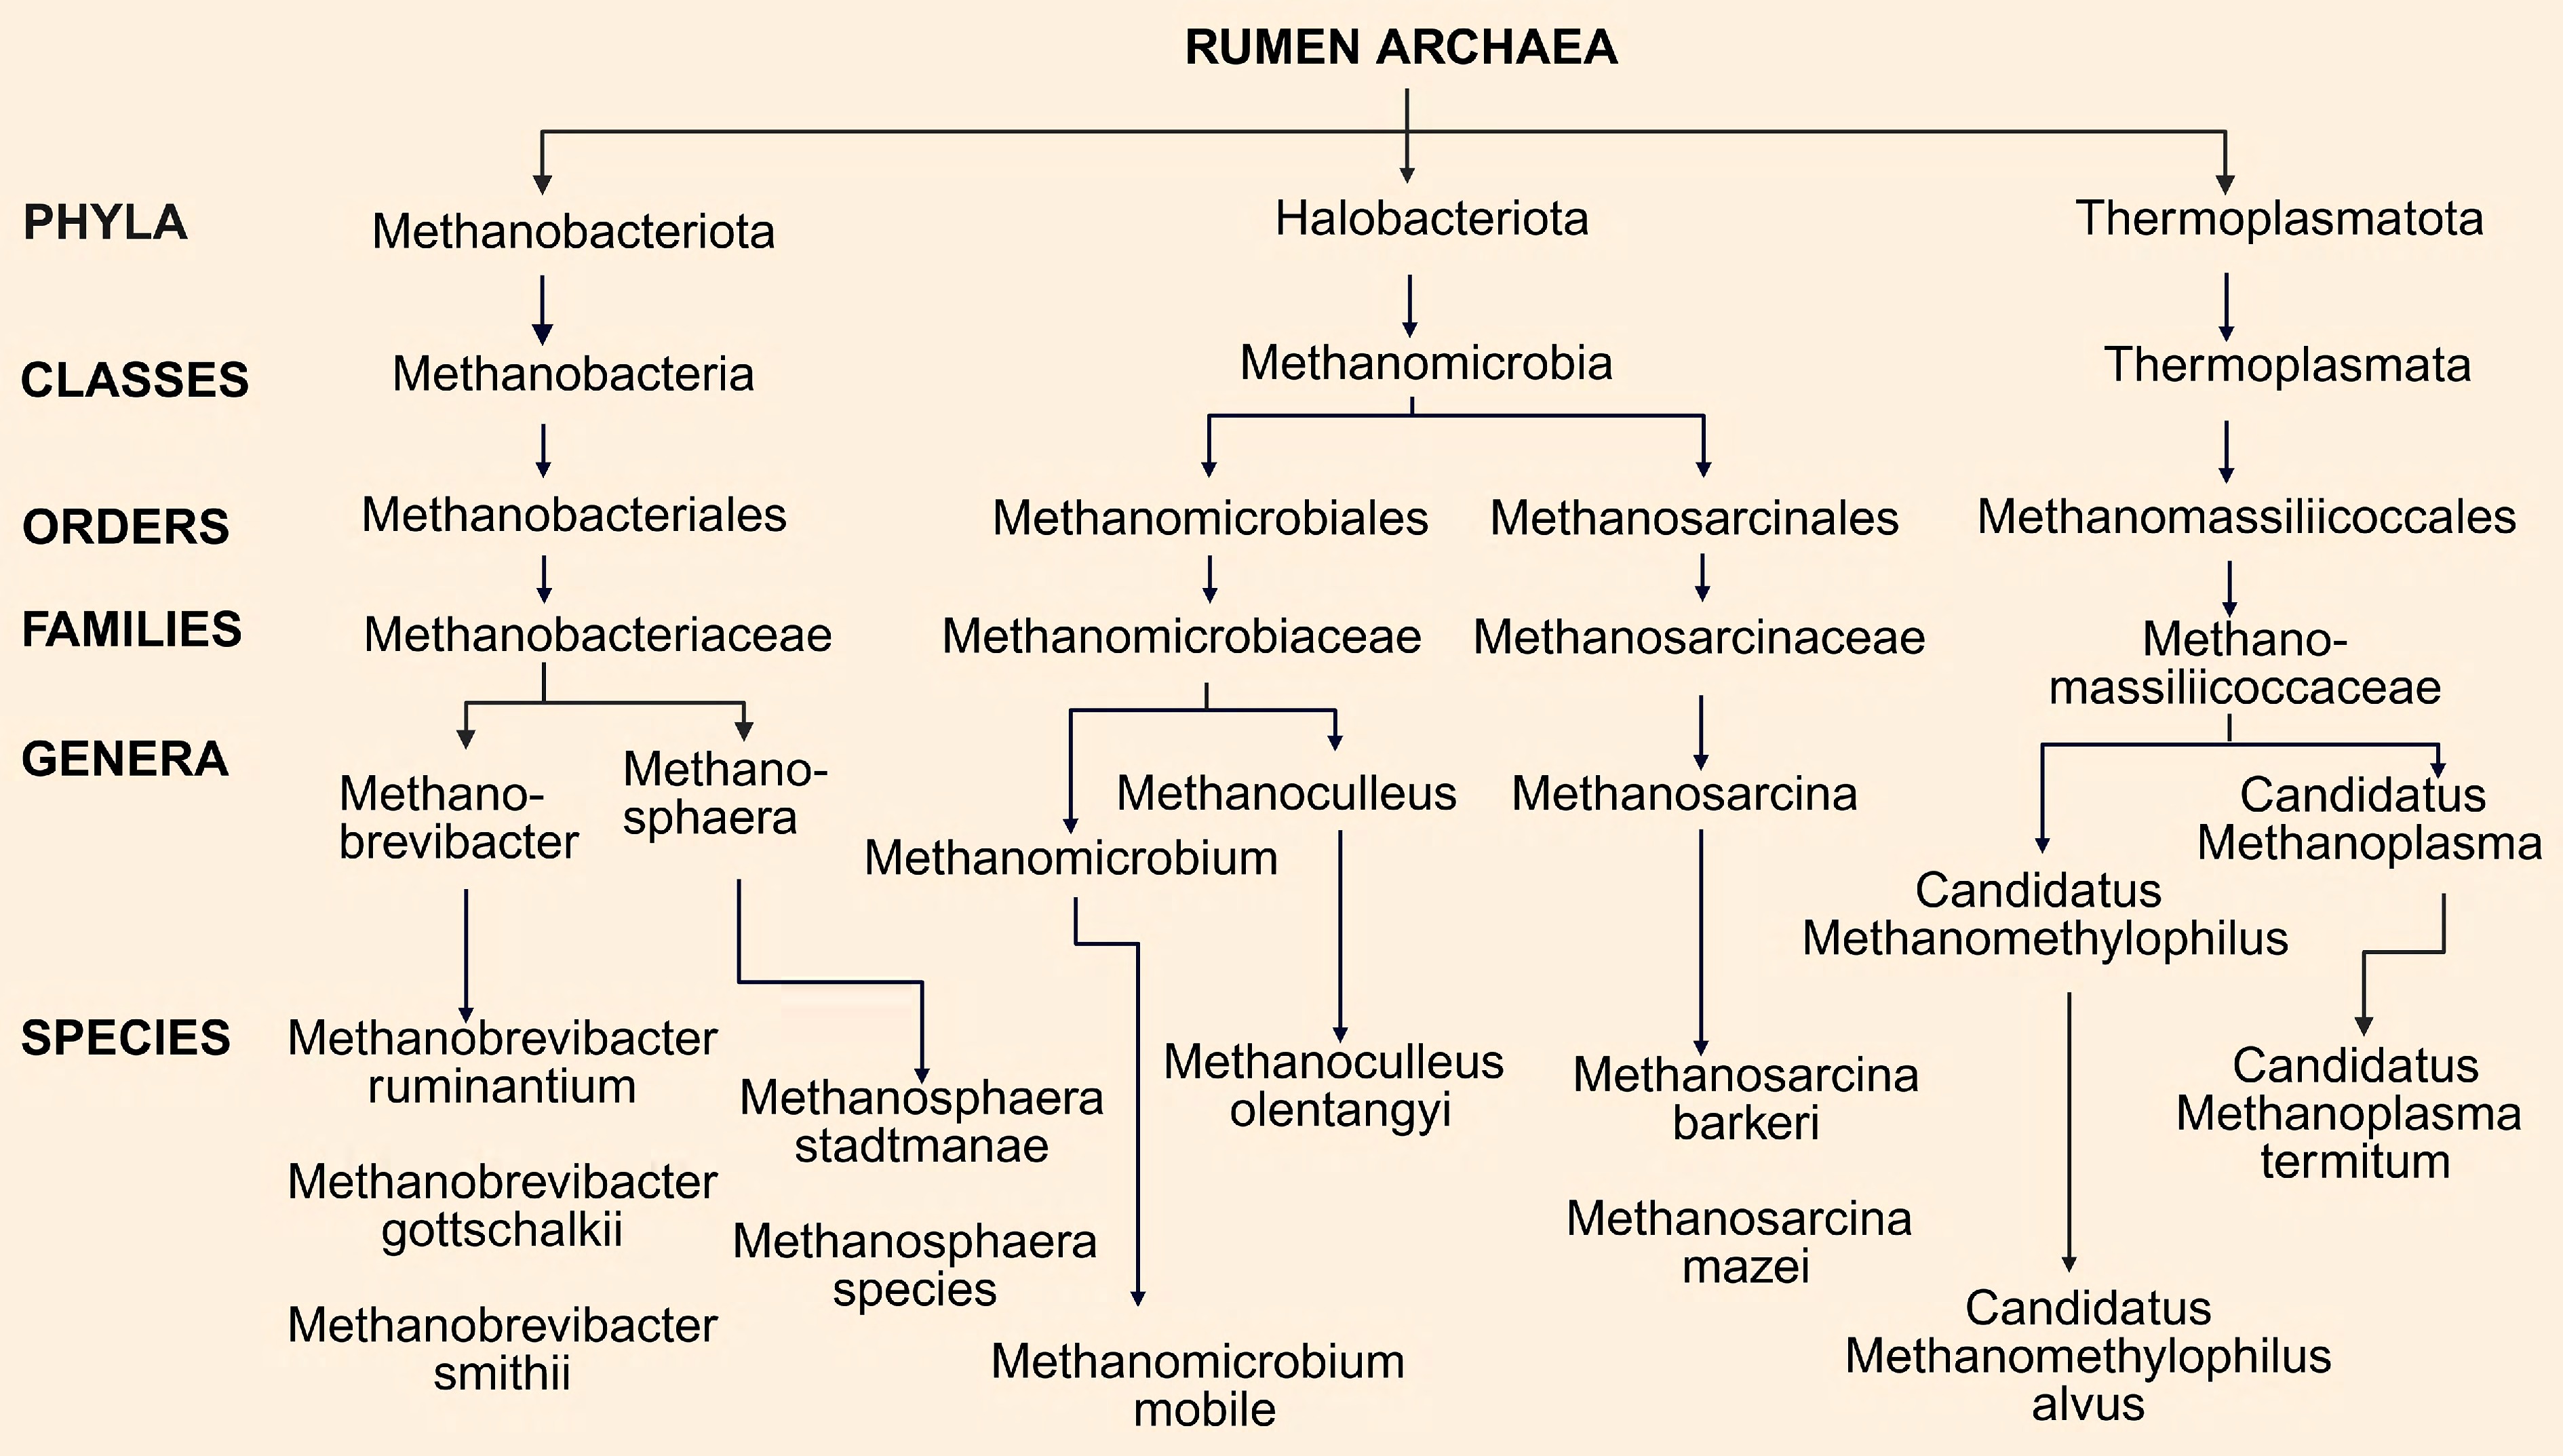
Figure 1.
Classification of methanogenic archaea.
Biochemical pathways of methanogenesis
-
The major biochemical pathways involved in the rumen methanogenesis are summarized in Fig. 2. During fermentation of complex plant carbohydrates, electrons are transiently captured by carriers such as NAD+, NADP+, and ferredoxin[21,22]. These reduced carriers help to maintain redox balance and support fermentation by transferring electrons to oxidized intermediates or protons (H+) in the presence of microbial hydrogenases, resulting in the formation of molecular H2, 70%−80% of which is used in methanogenesis[23,24]. Among the methanogenic pathways, the hydrogenotrophic pathway is the predominant one; it uses H2 and CO2 or formate as substrates and contributes to 70%−90% of enteric CH4 production[25,26]. Initially, CO2 binds to methanofuran (MF) and is reduced to formylmethanofuran (formyl-MF) by formyl-MF dehydrogenase using reduced ferredoxin as an electron donor[27]. Subsequently, the formyl group is transferred via formyltransferase to tetrahydromethanopterin (H4MPT), forming formyl-H4MPT. The intermediate is dehydrated and reduced to methyl-H4MPT, using reduced coenzyme F430 as an electron donor, and enzymes including methylenetetrahydromethanopterin dehydrogenase, methenyl-H4MPT cyclohydrolase, and 5,10-methenyl tetrahydro-methanopterin reductase[28]. The methyl group from methyl-H4MPT is then transferred to coenzyme M (HS-CoM) to form methyl-coenzyme M (methyl-S-CoM) with the help of methyltransferase. Methyl-S-CoM reacts with HS-CoM to produce CH4 with the help of the enzyme methyl-coenzyme M reductase (MCR)[29]. Acetate serves as the major substrate in the acetoclastic pathway, and its conversion to acetyl-CoA requires ATP, coenzyme A, acetate kinase, and phosphotransacetylase. The acetyl-CoA is further degraded by the CO2 dehydrogenase/acetyl-CoA synthase complex; its methyl group attaches to the corrinoid iron-sulfur protein and then to H4MPT, forming methyl-H4MPT. Methanol, methylamine (mono-, di-, or trimethylamine), or methyl sulfides are the substrates of the methylotrophic pathway[30]. The methyl group of the substrate attaches to a specific corrinoid protein via Mtr enzymes. The methyl group then binds to the HS-CoM, forming methyl-CoM to produce CH4[31].
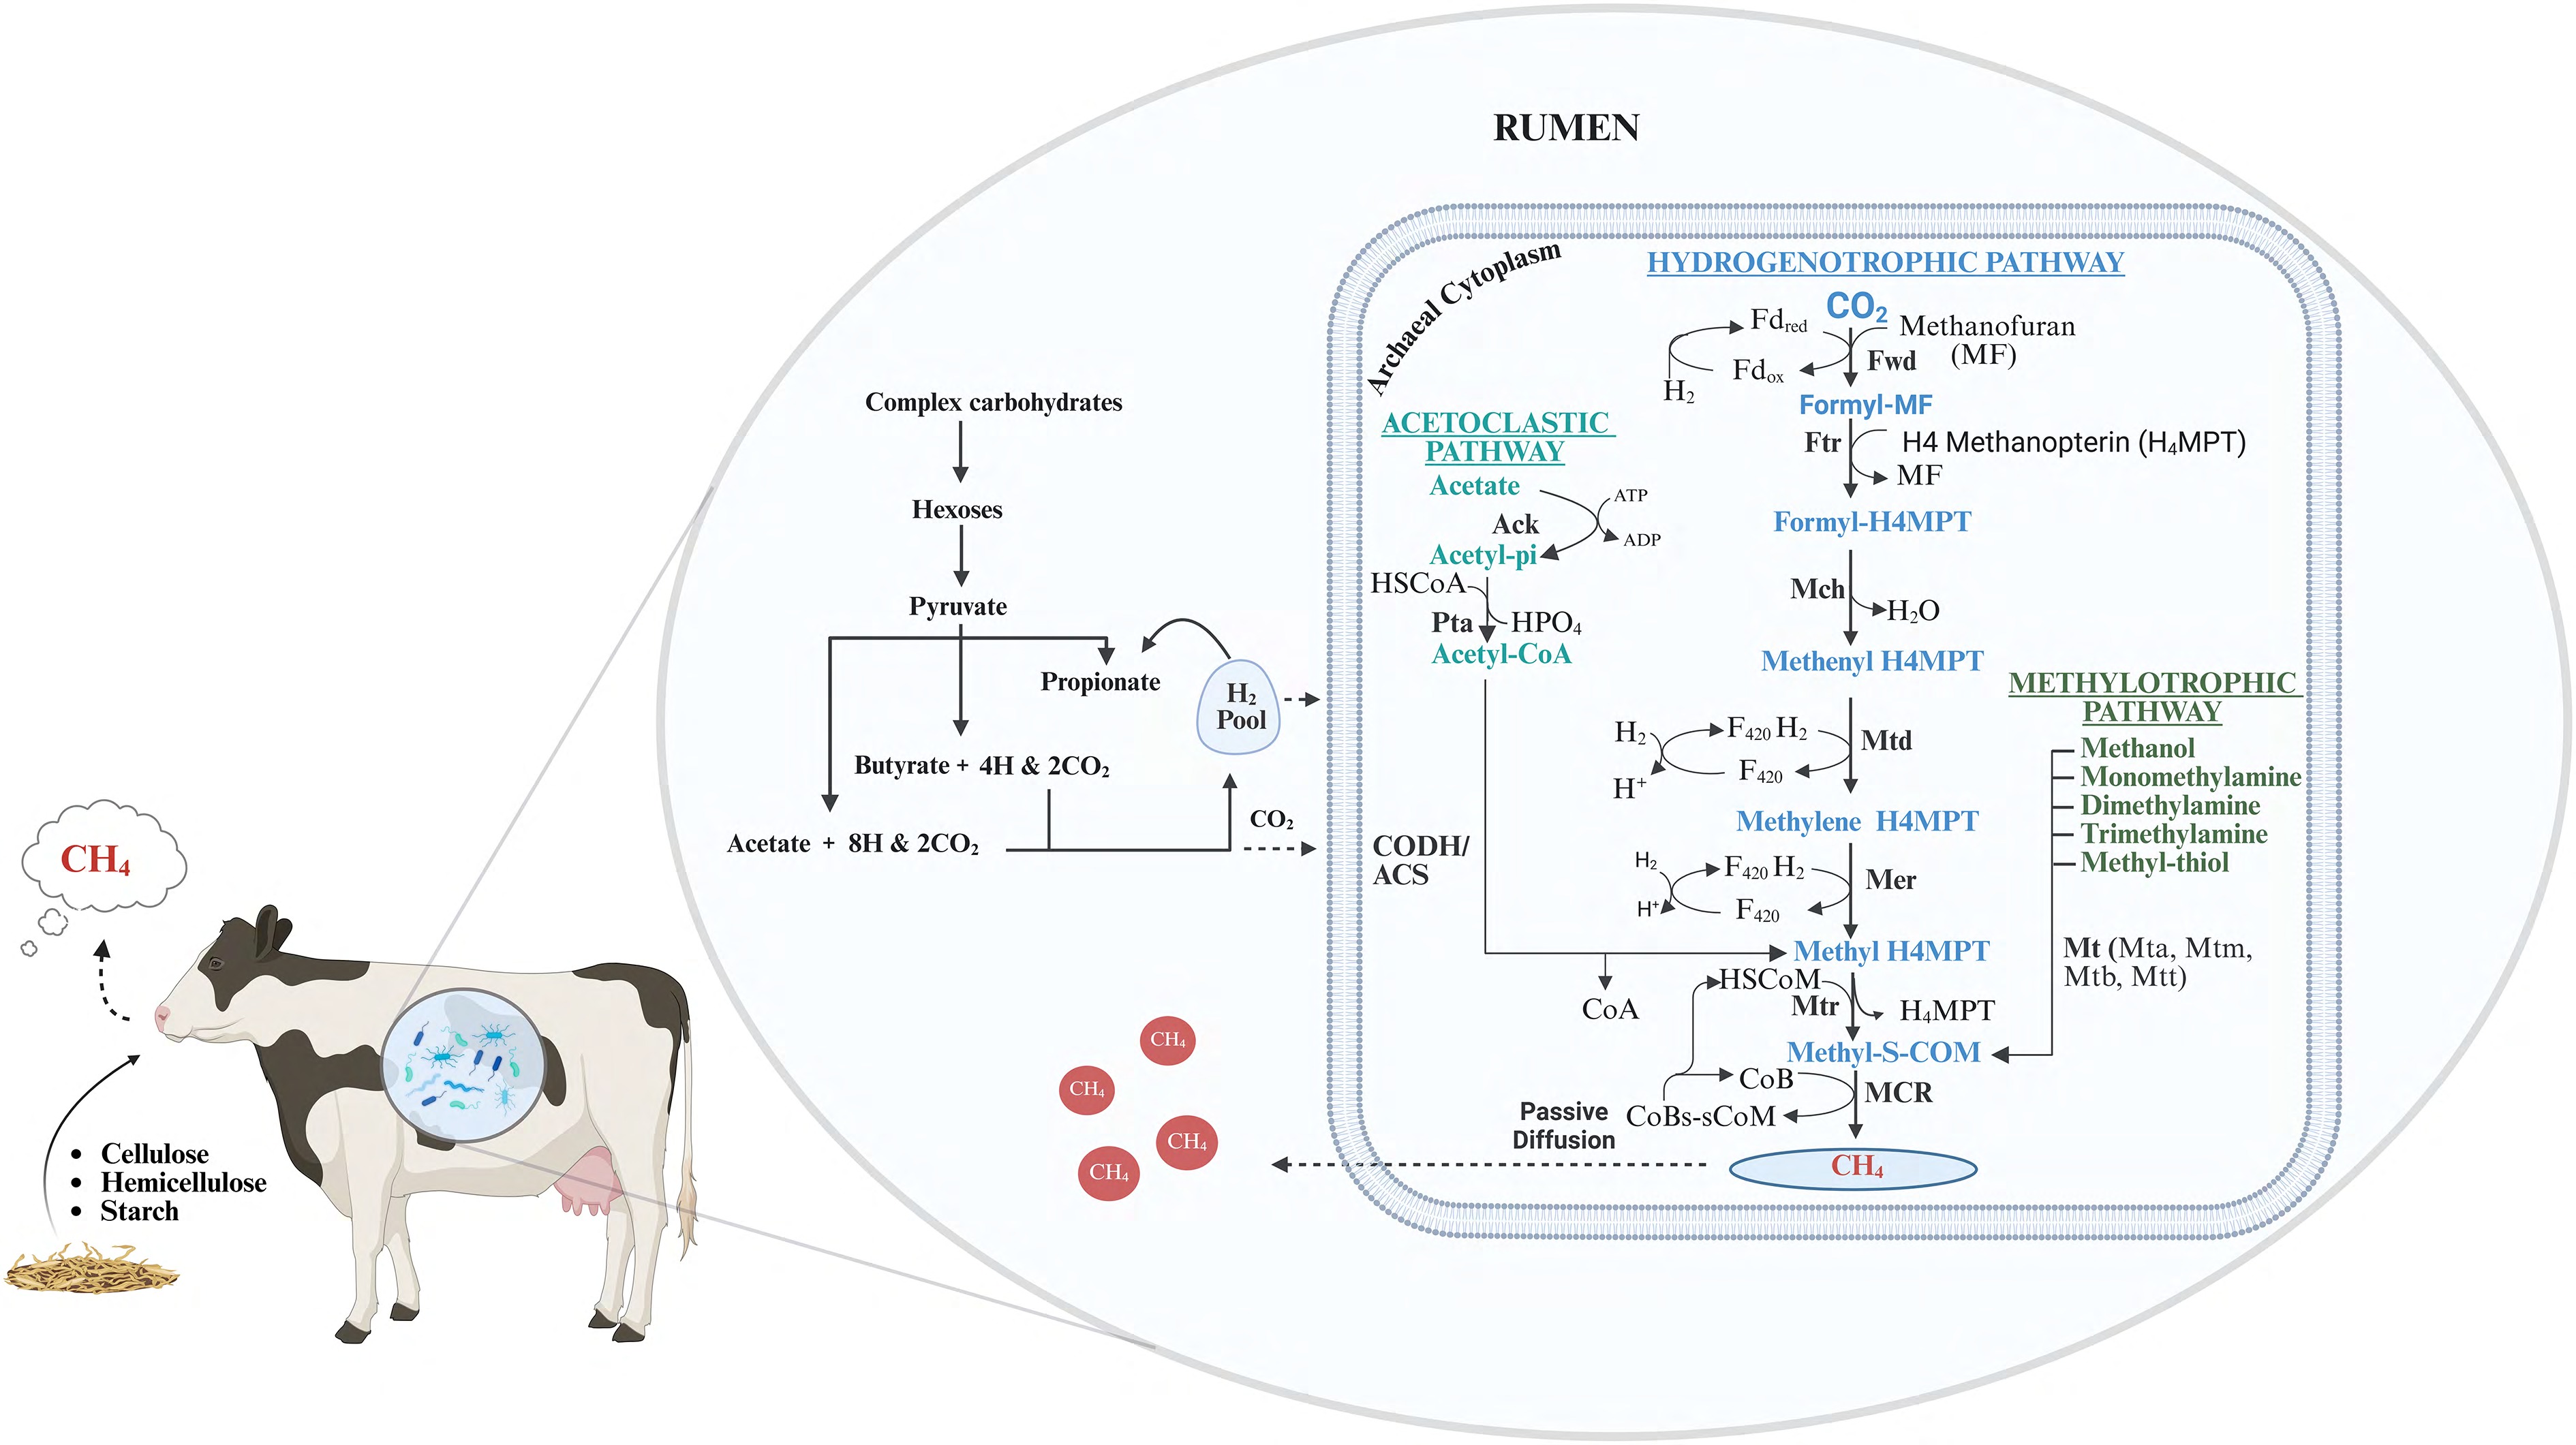
Figure 2.
Major biochemical pathways involved in the rumen methanogenesis (adapted from reference[20]). Abbreviations: Ack, acetate kinase; ACS, acetyl-CoA synthase; ATP, adenosine triphosphate; CH4, methane; CODH, carbon monoxide dehydrogenase; CoA, coenzyme A; CoB, coenzyme B; F430, cofactor F430; Fd, ferredoxin; Ftr, formyltransferase; H4MPT, tetrahydromethanopterin; Mer, methylene-H4MPT reductase; MF, methanofuran; Mch, methenyl-H4MPT cyclohydrolase; Mtd, methylene-H4MPT dehydrogenase; Mtr, methyl-H4MPT:coenzyme M methyltransferase; Mt (Mta, Mtm, Mtb, Mtt), methyltransferases; Pta, phosphotransacetylase.
-
The first chemical synthesis of 3NOP is reported in a previous study[32]. Briefly, 3NOP is produced by esterification of a three-carbon alcohol (propanol or 1,3-propanediol) with nitric acid, forming a nitrate ester (−ONO2), and the product is purified to yield stable 3NOP. The CH4 reducing capacity of 3NOP was first discovered in the Clean Cow project initiated in 2007 by Royal-DSM, and its description was publicly reported at the American Dairy Science Association meeting in 2014. The molecular formula of 3NOP is C3H7NO4; it is a colorless, water-soluble liquid with a slightly sweet odor. Its molecular weight is 121.09 g/mol, density 1.12 g/cm3, boiling point 120 °C, and melting point is −20 °C. Structurally, 3NOP consists of a 3-carbon chain (propanol), with a hydroxy group (OH) at the first, and a nitro group (NO2) at the third carbon, forming a nitrate ester (−O-NO2)[33].
Mode of action of 3NOP
-
3NOP inhibits the activity of the MCR, the key enzyme of the final step of methanogenesis (Fig. 3). MCR consists of α, β, and γ subunits with a nickel (Ni)-containing tetrapyrrole cofactor, F430, at its active site. For enzymatic activity, the Ni ion must be in the Ni1+ oxidation state[28,34]. The cofactor F430 (Ni2+)/ F430 (Ni1+) redox couple has a potential of approximately −600 mV, making Ni a strong reducing agent, which is highly sensitive to the oxidants[35]. Under normal conditions, Ni1+donates an electron to the methyl–S–CoM, forming a methyl radical, converting Ni1+ to Ni2+. The methyl radical then reacts with the thiol group of HS-CoB to produce CH4, and the rest of the thiyl radicals of CoM and CoB rejoin together to form a heterodisulfide bond (CoM-S-S-CoB). This bond is then recycled to thiol forms, and Ni1+ is oxidized to Ni2+ to re-establish the MCR activity. The enzymatic degradation of 3NOP can lead to the production of oxidants like nitrate or nitric oxide-related radicals. These radicals react with the Ni1+ center of F430 and oxidize it to Ni2+. Consequently, Ni is no longer able to donate an electron to methyl-CoM, thus inhibiting the formation of methyl radicals and inhibiting CH4 production[35,36].
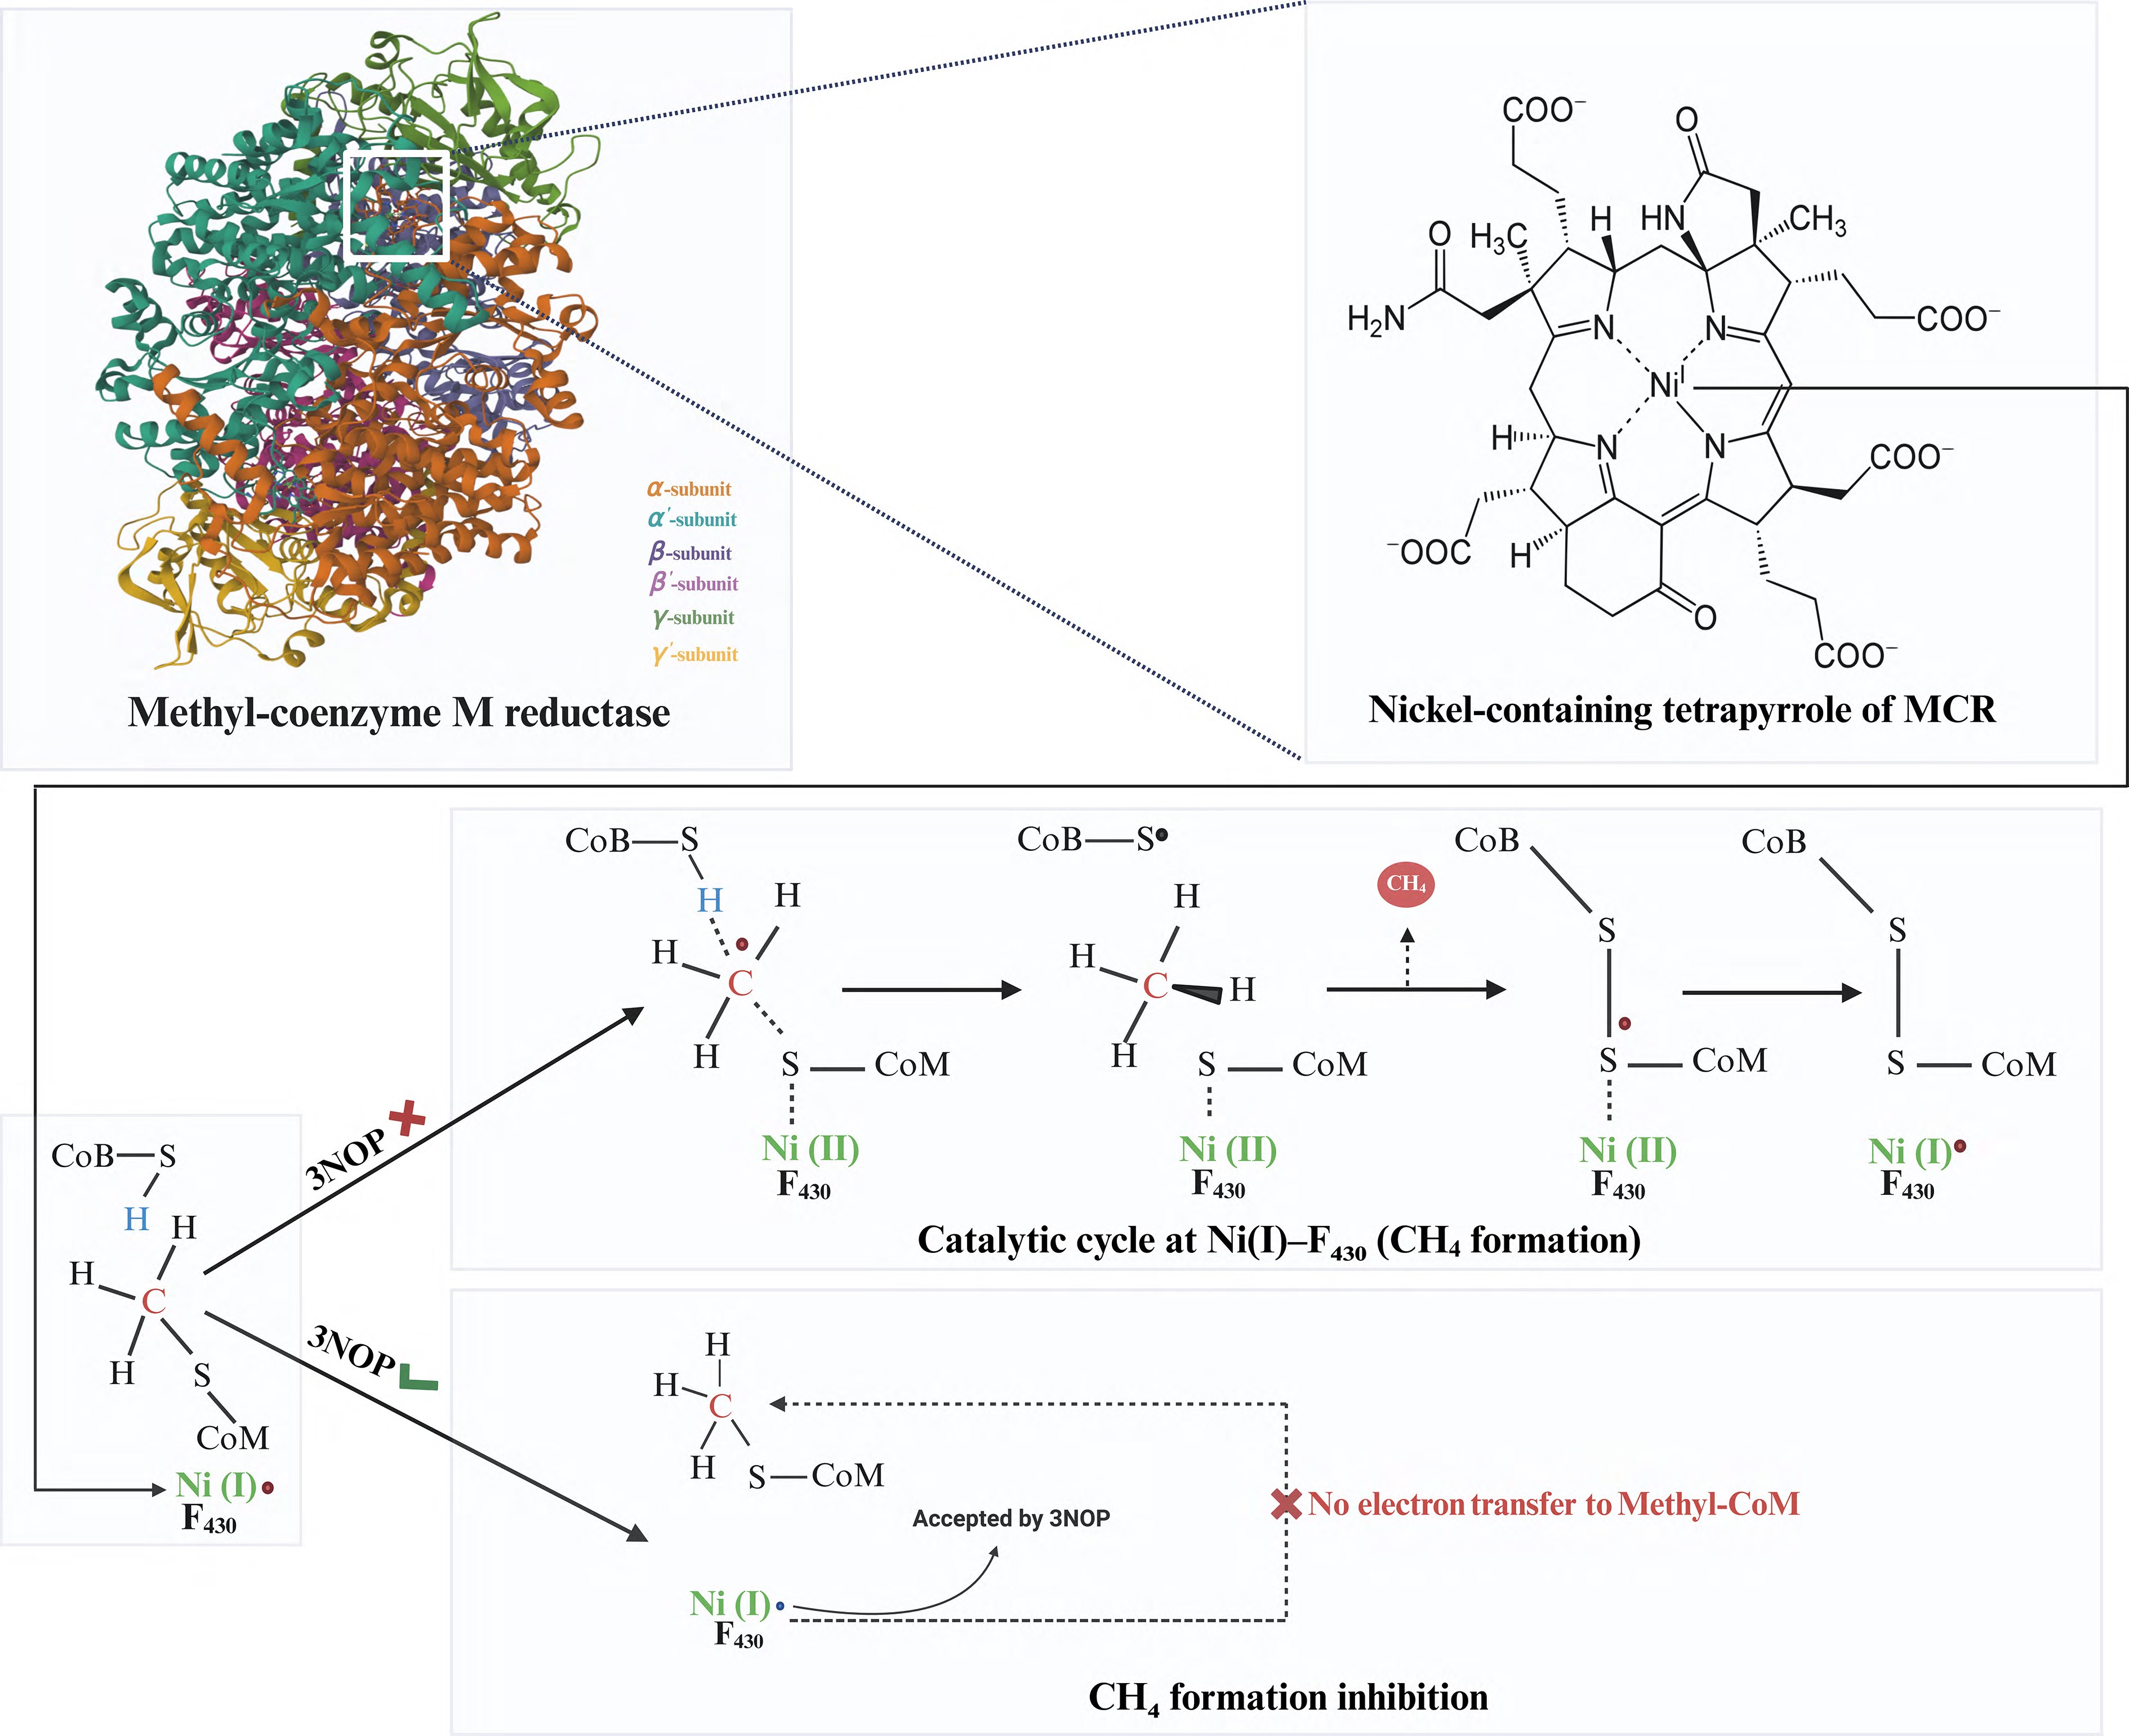
Figure 3.
Three-dimensional structure of MCR, highlighting the nickel-containing active site and the inhibitory mechanism of 3NOP (adapted from the study by Shima et al.[37]).
Metabolism and safety of 3NOP
-
In the rumen, the nitrate ester bond of 3NOP is rapidly hydrolyzed by microbial action, producing metabolites like 1,3-propanediol and inorganic nitrate/nitrite. 1,3-propanediol is transformed into 3-hydroxypropionic acid (HPA)[38]. In an alternative way, 3NOP is first oxidized to 3-nitrooxypropionic acid (NOPA), which is then hydrolyzed to HPA and inorganic nitrate[11,39]. NOPA is a plasma metabolite, while HPA is utilized in mammalian cells as a substrate for acetyl-CoA and propanoyl-CoA synthesis[39]. The core metabolic pathway of 3NOP remains remarkably consistent across different species and experimental conditions. However, the rate and metabolic fate of the intermediates differ among species, physiological states, rumen environment, diet composition, and feeding pattern[39−42]. Trace quantities of 3NOP or its intermediates (e.g., NOPA) may enter systemic circulation; however, studies have reported no toxic residue accumulation in blood, milk, liver, muscle, or meat[33,39,43]. Moreover, key blood metabolites and liver enzymes, including glucose, urea, β-hydroxybutyrate, non-esterified fatty acids (FA) glutamyl transferase, alkaline phosphatase, alanine aminotransferase, and aspartate aminotransferase, remained within normal ranges, indicating no adverse effects on animal health[44,45]. Both EFSA and the Food Safety Commission of Japan (FSCJ) concluded that Bovaer® is safe at recommended inclusion levels. EFSA considered broader aspects such as animal safety, user exposure, and environmental impacts, while FSCJ mainly focused on consumer food safety[11,46]. However, in late 2025, Danish farmers reported health complications like diarrhea, fever, reduced milk yield, digital dermatitis (hoof infections), elevated somatic cell counts, reproductive disorders, and even mortality in some cases in dairy cattle following the use of Bovaer®[47]. Therefore, despite the established safety profile and regulatory approvals, recent field reports of health issues necessitate further investigation into the long-term effects of 3NOP, including high-dose exposure and its impacts across diverse production systems.
-
In dairy cattle, the reported CH4 reduction ranges from 21%−64.5% in terms of daily production (g/d), and 21%−59.5% in terms of dry matter intake (DMI; g/kg), at dosage ranging from 40−200 mg/kg DMI[48−50]. Similarly, in beef cattle, CH4 reduction ranges from 22%−90% (g/d) and 22%−87.6% (g/kg DMI) at 50−325 mg/kg DMI dose range[42,51,52]. However, some studies have reported lower (< 20%) mitigation responses[53−55]. These studies have demonstrated that 3NOP efficacy is highly influenced by the dose rate, diet composition, production system, and dosing method. A qualitative synthesis of the studies, as summarized in Tables 1 and 2, indicates a clear dose-dependent response of 3NOP supplementation. At low inclusion levels (< 60 mg/kg DMI), CH4 mitigation is generally modest, typically ranging from 8%−25% (g/kg DMI). Moderate doses (60−100 mg/kg DMI), which represent the most frequently tested range in dairy and beef cattle, consistently achieved 20%−40% (g/kg DMI), reductions in CH4 emissions. At higher inclusion levels (> 100 mg/kg DMI), CH4 emissions are typically reduced by 50%−80% (g/kg DMI), although the response tends to plateau beyond certain dose levels. Diet composition also influences the mitigation response. Under high-forage diets, CH4 reductions are generally moderate, approximately 10%−35% (g/kg DMI), whereas under high-concentrate (HF) diets, 3NOP shows stronger inhibition, with reductions frequently exceeding 40% and occasionally reaching 60%−80% (g/kg DMI), particularly at higher inclusion levels of 3NOP. An increase in H2 emissions with 3NOP supplementation is consistently reported, although the actual emissions are lower than theoretically expected[56,57]. For example, a 162 g/d CH4 reduction should have spared approximately 40.7 g of H2, but only 1.27 g/d of H2 was emitted, suggesting its redirection towards alternative metabolic sinks[54,58]. Similarly, some studies reported increases in CO2 production with 3NOP[50,59]. In conclusion, 3NOP is consistently reducing CH4 emissions and can redirect H2 towards alternative metabolic pathways, which can enhance rumen fermentation efficiency.
Rumen pH
-
The use of 3NOP has also been reported to increase rumen pH[60,61]. This rise is probably due to a decline in the relative concentration of volatile fatty acids (VFA), accompanied by an increase in butyrate levels. Butyrate can remove an additional proton, which contributes to the rise in rumen pH[62]. Moreover, interaction effects of dose and diet on the rumen pH have been documented, where 3NOP supplementation with high fiber diets was associated with an increase in rumen pH[63]. Similarly, higher dose (2,500 mg/d) is reported to increase rumen pH as compared to lower doses (500 mg/d)[53]. In conclusion, 3NOP supplementation is likely to increase rumen pH, though its magnitude depends on the dose and diet.
Volatile fatty acid profiles
-
Multiple studies, as shown in Tables 1 and 2, have reported an increase in propionate, butyrate, and valerate levels with a reduction in acetate, acetate-to-propionate ratio, and total VFA, with 3NOP supplementation[55,60,64−66]. The composition of the diet also affects the VFA profile; for example, high-starch diets stimulate propionate production, whereas high-fiber diets suppress propionate production[57,67−69]. In short, 3NOP can produce a consistent effect on rumen fermentation profiles, favoring the production of propionate and butyrate, while inhibiting the production of acetate.
Ammonia-N concentration
-
A decrease in the ammonia-N (NH3-N) concentration with 3NOP supplementation is reported by several studies[57,70,71]. It is an indication of enhanced utilization of dietary nitrogen[72]. This response may stem from increased ruminal H2 partial pressure following the inhibition of methanogenesis; this elevation can suppress amino acid deamination and proteolysis, thereby reducing ammonia production and promoting microbial nitrogen incorporation[65,73]. Similarly, a low NH3-N concentration accompanied by reduced butyrate levels was reported, presumably when the rumen fluid was sampled 2 h before feeding; a period associated with the least microbial activity and NH3 production[57], unlike past studies in which rumen fluid was sampled 3 to 4 h post-feeding[74]. Overall, 3NOP lowers NH3-N levels, which indicates better nitrogen utilization, but sampling time and fermentation dynamics may affect it.
Rumen microbial community structure
-
3NOP supplementation consistently inhibits hydrogenotrophic methanogens, especially those belonging to the order Methanobrevibacter and Methanomassiliicoccaceae, while methylotrophic taxa usually persist or show a transient increase[70,75−77]. These suppressions were confirmed by 56% reductions in methanogen 16S rRNA gene copies, and a 5.6-fold decrease in mcrA transcript abundance[51,78]. 3NOP also suppresses fibrolytic and acetate-producing bacterial taxa such as Ruminococcus, Clostridium, Sarcina, and members of Lachnospiraceae and Ruminococcaceae, while enriching butyrate- and propionate-producing genera like Butyrivibrio, Succiniclasticum, Succinivibrionaceae, Prevotellaceae, and Fibrobacter[75,77−79]. Diet-linked suppression of methanogens under high-grain diets and distinct bacterial enrichments based on substrate availability have been reported[77]. Protozoal and fungal communities appear relatively resilient to 3NOP supplementation. Major rumen ciliate groups, including Entodiniomorpha and Holotricha, generally remain unchanged[71,80], although some modest increases in certain genera, such as Epidinium and Entodinium, have occasionally been reported[65,76,78]. Similarly, rumen anaerobic fungi show no significant changes[81]. Supplementation of 3NOP in young calves can induce long-term microbial shifts, which were reported to maintain CH4 reductions even after withdrawal, indicating the possibility of a long-term rumen microbial programming strategy[76,82]. Collectively, 3NOP selectively suppresses the activities of methanogenic archaea and does not affect the functional stability of bacterial, protozoal, and fungal communities.
Table 1. Effects of 3NOP supplementation on CH4 emission, H2 production, and rumen fermentation in ruminants.
Animal type Diet 3NOP dose
(mg kg/DMI)CH4 yield
(g/kg DMI) (△%)H2 fold change Volatile fatty acids Ref. Acetate (△%) Propionate (△%) A:P ratio (△%) Dairy cow F:C (63:37) 60 ↓46 ↑4.2 ↓7.7 ↑6.6 (T) ↓14.9 [83] Dairy Cow PMR-based diet 80 ↓26−28 ↑2.7−2.8 − − − [84] Dairy Cow F:C (68:32) 60 ↓11−21.8 ↑2.5−3.7 − − − [85] Dairy Cow F:C (56:44) 60, 80 ↓31−34 − − − − [86] Dairy Cow F:C (60:40) 68, 132 ↓23−60 − − − − [77] Dairy Cow Grass silage 80 ↓22 ↑4.4 − − − [87] Dairy Cow Grazing 80 ↓28.5 ↑1.6 − − − [88] Dairy Cow Grazing 130 ↓9.7−10.2 ↑1.6 ↓5.7 ↑11.8 ↓14.7 [55] Dairy Cow F:C (53:47) 80 ↓23 − − − − [43] Dairy Cow F:C (76:24, 81:19, 65:35, 75:25) 80 ↓20 ↑3.3 − − − [50] Dairy Cow F:C (70:30) 60 ↓8−18 ↑1.53−2.85 − − − [89] Dairy Cow F:C (60:40) with low or high-fat 80 ↓24 ↑36 ↓8.5 ns ↓7.2 (T) [90] Dairy Cow F:C (53:47) 80 ↓18−23 ↑3.54 − − − [91] Dairy Cow Plant protein or urea-based 100 ↓53.5 − ↓5 ↑23 ↓25 [92] Dairy Cow F:C (60:40) 60 ↓26−30 − ↓10 ns ↓10 [75] Dairy Cow Grass or corn silage 60, 80 ↓30.9−35.9 ↑3.7−4.7 − − − [59] Dairy Cow LC (30%) and HC (55%) 48, 51 ↓23−35 − ↓4.9 ↑9.3 ↓15 [71] Dairy Cow F:C (58:42) 60 ↓21 ↑6 − − − [56] Dairy Cow F:C (60:40) 40–200 ↓16−36 ↑6−10 − − − [93] Dairy Cow F:C (58:42) 60 ↓27 ↑6 − − − [49] Dairy Cow F:C (60:40) 60 ↓16 ↑12 − − − [94] Dairy Cow S:C (66:34) 100 ↓21−23 − − − − [95] Dairy Cow S:C (60:40) 66.5, 133 ↓23−37 − ↓9.9 ↑10.9 ↓18.7 [80] Dairy Cow F:C (55:45) 60 ↓34 − ↓6.1 ↑5.2 ↓11 [70] Dairy Cow F:C (54:46) 40, 60, 80 ↓25−32 − − − − [54] Dairy Cow F:C (38:62) 130 ↓60 − ↓6.1 ↑10.5 (T) ↓14.4 [48] Dairy Cow Maize silage-based 25, 124 ↓7−9.8 − ↓6.3 ↓8.9 ↑9.7 [53] Beef cattle F:C (83:17) 121 ↓19.4 ↑4.21 − − − [96] Beef Cattle F:C (90:10) 200 ↓31.6−51.4 − − − − [81] Beef Cattle F:C (10:90) 100 ↓38 ↑3.73 − − − [45] Beef Cattle F:C (50:50) 150 ↓27.2 ↑3.27 − − − [57] Beef Cattle F:C (11:89) 100, 150 ↓40.7 − − − − [97] Beef Cattle F:C (90:10) 150 ↓22.0 ↑320 ↓7.9 ↑13.5 ↓18.9 [52] Beef Cattle F:C (3:97) 0, 50, 75, 100, 125 ↓65.5−87.6 − − − − [42] Beef Cattle F:C (90:10) 200 ↓28.2 ↑37.5 ↓8 ↑18 ↓25 [98] Beef Cattle F:C (90:10) 200 ↓36.6 ↑46 ↓11.5 ↑16.5 ↓22 [68] Beef Cattle F:C (89:11) 100, 125, 150 ↓52−76 ↑1.9 ↓8 ↑23 ↓30 [99] Beef Cattle S:C (70:30) 150, 175, 200 ↓20−25 ↑3.5−4 − − − [100] Beef Cattle F:C (90:10) 150 ↓53 ↑8.8 − − − [101] Beef Cattle S:barley grain (92:8) 125 ↓70 − − − − [102] Beef Cattle F:C (65:35) 100 ↓18 − ↓7.8 ↑13.5 ↓18.7 [63] Beef Cattle Rhodes grass hay 325 ↓38 − − − − [51] Beef Cattle S:C (65:35, 8:92) 125, 200 ↓37−42 ↑89 ↓9.4 ↑15.5 ↓19.5 [103] Beef Cattle S:C (65:35, 8:92) 50, 75, 100, 150, 200 ↓23−45 − − − − [104] Beef Cattle S:C (70:30, 8:92) 100, 200 ↓16−45.2 ↑2.6–621.5 − − − [105] Beef Cattle F:C (60:40) 280 ↓59.2 − ↓9 ↑19.9 ↓25 [78] Sheep F:C (70:30) 80−120 ↓11.8−14.7 ↑3.1−11.8 − − − [106] Sheep F:C (60:40) 55, 623 ↓21.7−22.1 − ↓6.8 ↑22.4 ↓20.4 [107] CH4: methane; H2: hydrogen; (△%): treatment response over control; ns: not-significant; ↓: decreased; ↑: increased; −: not reported; DMI = dry matter intake; A:P ratio: acetate to propionate ratio; DW: drinking water; DM: dry matter; T: numerical tendency (p > 0.05); F:C: forage to concentrate ratio; S:C: silage to concentrate ratio; B: Bovaer®; fold change: control vs 3NOP. Table 2. Summary of in-vitro studies on the effects of 3NOP on CH4 emissions, H2 production, and rumen fermentation.
Rumen fluid Diet 3NOP (mg/g OM) CH4 yield
(g/kg DMI) (△%)H2 fold change Volatile fatty acids Ref. Acetate (△%) Propionate (△%) A:P ratio (△%) Cattle F:C (56:44) 2, 2 (Vita B12) ↓9−12 − ↓2.60 ↑2.55 ↓4.79 [108] Cattle F:C (56:44) 2, 100 (Fumarate) ↓9.7−11.5 − ns ns ↓3.6 [79] Cattle F:C (70:30, 40:60) 0.07, 0.16, 1.2 ↓17−97 ↑27−6.2 ↓4 ns ns [109] Cattle F:C (50:50) 0.08 ↓44 − ↓5.5 ↑7.1 ↓13.6 [110] Cattle S:C (60:40) 0.5 ↓75 ↑1.81 ↓15.8 ↑10.2 (T) ns [111] Cattle S:C (60:40) 0.5, 1, 2 ↓74.6−86 ↑2.6−3.18 − − − [112] Sheep F:C (60:40) 0.025, 0.05, 0.1 ↓97 ↑484 ↓15.8 ↑5.9 ↓15.2 [66] Sheep Alfalfa hay and oats 8, 16 ↓86−95.4 − − − ↓33.1 [107] CH4: methane; H2: hydrogen; (△%): treatment response over control; ns: not-significant; ↓: decreased; ↑: increased; −: not reported; T: numerical tendency (p > 0.05); OM: organic matter; A:P ratio: acetate to propionate ratio; F:C: forage to concentrate ratio; S:C: silage to concentrate ratio; fold change: control vs 3NOP. -
It has been demonstrated that CH4 emissions decrease with increases in 3NOP doses[54,65]. A 2.82% (g/d) and 2.26% (g/kg DMI) decrease in yield, and a 2.75% decrease in the intensity (g/kg of milk yield) of CH4 emissions with each 10 mg/kg DM increase in 3NOP dose was reported[69]. Nearly similar reductions ranging from 2.56% (g/d) and 2.48% (g/kg DMI) in CH4 yield with each 10 mg/kg DM increase in 3NOP dose were previously reported[67]. However, after approaching a certain threshold level, the response to further increases in the 3NOP dose begins to plateau. This plateau effect has been consistently observed in both beef and dairy cattle[93,113]. Dairy and beef cattle have a recommended average dosage rate of 60−100 and 100−150 mg/kg DMI, respectively[46]. Dose optimization under regulatory limits is required to maximize the CH4 reduction and to avoid the negative effects of higher doses on animal health and productivity.
Diet composition
-
Methane emissions decrease with supplementation of 3NOP under a variety of basal diets such as grass silage (GS), corn silage (CS), grass-corn silage mixture (GSCS), HC, and low concentrate (LC) diets, but the extent is more pronounced with CS, GSCS, and HC diets[59]. This is likely because of higher starch and lower neutral detergent fiber (NDF) concentrations in these diets. An increase in dietary starch levels has been reported to decrease CH4 emissions[114]. Direct comparisons of the above diets revealed that GSCS and CS have starch concentrations of 154, and 212 g/kg DM, respectively, which were higher compared to the GS-based diet (98 g/kg DM)[59]. Greater starch concentration in the diet promotes propionate formation, lowers rumen pH, and inhibits methanogens, thereby enhancing 3NOP efficacy[115]. Increases in dietary NDF levels can decrease 3NOP efficacy, as meta-analyses have evidenced it by reporting a 0.6%−1.5% decrease in 3NOP efficacy with every 10 g/kg DM increase in NDF concentration[67,69,113]. Similarly, an increase in the NDF levels beyond 31.8% in the diet significantly reduces 3NOP efficacy[116]. Higher dietary fat also reduces 3NOP efficacy, where each 10 g/kg DM decrease in the fat content of the diet increases CH4 reduction by 3.1%. Similarly, every 10 g/kg DMI increase in urea reduces the efficacy of 3NOP by 0.71%. Conversely, every 10 g/kg increase in dietary CP content above 14.5% DM level enhances the efficacy of 3NOP by 0.63%[69,116]. In summary, 3NOP efficacy is strongly dependent on diet composition, with greater efficacy being reported for starch-rich diets, while higher concentrations of fat, NDF, and urea diminish its effectiveness.
Ruminant species and breeds
-
The species- and breed-specific differences are also reported by some studies. Under similar supplementation levels (e.g., 500 mg/kg DMI), CH4 reductions in dairy cattle was 6.6%, while in sheep it was 29%[51,53]. Similarly, 3NOP efficacy across different cattle types also varies, as greater responses in dairy cows are reported occasionally, possibly due to their higher mean DMI (22.3 ± 4.13 vs 7.3 ± 0.97 kg/d in beef cattle)[67,117]. However, beef cattle tended to show greater percentage reductions with 3NOP supplementation relative to their control. Notably, cattle type is less important than diet composition and 3NOP dosage[116]. An 18% (g/d) CH4 reduction in Holstein Friesian and 8% (g/d) in Brown Swiss cattle under a similar diet and dose was reported, highlighting breed-specific responses[89]. These differences were probably due to host genetics and rumen microbiome composition, such as the abundance of methanogenic archaea, which define the CH4-producing phenotype[118]. For instance, Methanobrevibacter were found to be more abundant in Holstein Friesian than in Brown Swiss cows[119]. In summary, species- and breed-specific differences affect 3NOP efficacy; hence, mitigation strategies in future must be designed to address these variations to achieve the desirable results.
Animal production stage and parity
-
In dairy cattle, 3NOP decreased CH4 emissions by 9%−16% in the dry period, 8%−29% in early lactation, 8%−17% in mid lactation, and 18%−23% in late lactation[50]. In-depth analysis revealed that these changes were predominantly related to dietary changes during the lactation phases. The relatively low mitigation impact during the dry period was associated with a high-forage (NDF) diet. In contrast, the highest mitigation during early lactation can be attributed to HC (starch) diets. Within each stage, CH4 reduction responses to 3NOP also varied. During mid lactation, reductions ranged from 17% (g/d) at the start to 8% (g/d) at the end, probably due to differences in diet composition[50]. 3NOP efficacy was found to be higher in multiparous cows than in primiparous cows. 3NOP supplementation reduced CH4 (g/kg DMI) by 35.3% in multiparous and 28% in primiparous cows at the same dose[91]. Overall, these findings show that basal diet composition is a stronger determinant of 3NOP efficacy than production stages.
Method of supplementation
-
The administration method has a strong impact on the effectiveness of 3NOP, as it determines its bioavailability and rumen residence time[63]. The most popular approach is mixing 3NOP with the total mixed ration (TMR), which guarantees uniform and continuous consumption. The effectiveness of this method, however, depends on the quality of feed mixing and the feeding behavior of the animal[48,52,67]. Top-dressing 3NOP on feed is based on voluntary consumption and generally has short-term effects (2 h post-feeding); unlike TMR-based delivery, it does not provide a continuous or evenly distributed intake[78]. Direct rumen infusion also causes short-term (1 to 2 h after administration) CH4 reduction, owing to the quick breakdown of 3NOP in the rumen[53]. On the other hand, the provision of 3NOP by drinking water to adult sheep has reduced CH4 emissions by 41.4% (g/d), which shows that water-based delivery is a viable solution, especially for pasture-based systems[106]. Therefore, in addition to dosage, the delivery method must also be considered in the quantitative evaluation of the CH4 mitigating potential of 3NOP[120]. Overall, the maximum efficacy of 3NOP can be achieved by adopting administration routes that allow its constant rumen presence, such as TMR mixing.
Timing and frequency of supplementation
-
3NOP is equally effective across the summer and winter seasons[83], however, timing and frequency of administration largely influence its efficacy[120]. A single 3NOP dose of 2.5 g/d was divided into three parts and administered at 0, 3, and 6 h after feeding, leading to a 38% (g/d) CH4 reduction[51]. In contrast, when the same nominal dose (2.5 g/d) is split into two equal portions and offered twice daily, the CH4 mitigation was only 9.8% (g/d)[53]. The greater reduction in CH4 can be related to the more frequent dosing and prolonged rumen exposure. Similarly, supplementation of 3NOP to grazing cows at milkings (twice daily), a 28.5% reduction (g/kg DMI) in CH4 emission within the first 3 h post-supplementation was noticed, with overall daily reduction only 5% (g/d), possibly due to the additive transient effect[88]. Therefore, dosing at regular intervals can enhance the 3NOP effectiveness.
Measurement technique
-
Respiration chamber system (RCS), sulfur hexafluoride tracer (SF6), and GreenFeed systems (GF) are commonly used for CH4 emission measurements. A meta-analysis study reported no significant differences in CH4 measured by the RCS or the SF6 techniques[63]. However, GF measured 8% less CH4 than SF6[54]. This discrepancy is likely due to the voluntary, visit-based sampling nature of GF, where animals may not visit the system during peak CH4 production (3 h post-feeding), whereas SF6 provides continuous sampling[121,122]. In short, CH4 measurement methods do not significantly alter the data on CH4 production.
Combination with other additives
-
Synergetic effects of 3NOP with other CH4-reducing additives have been reported in several studies. In feedlot cattle, supplementation of 3NOP has shown synergetic effects with canola oil and monensin, causing a marked reduction (up to 90%) in CH4 emissions (g/d). This potent effect of 3NOP was due to the enhanced CH4-suppressing environment created by the other additives[42]. Similarly, compared to 3NOP alone (31.6%), greater CH4 reduction (51%) was noticed for the 3NOP and canola oil combination[68]. However, these synergistic effects are not always consistent, as comparatively more modest reductions (41%) were noticed for the 3NOP-monensin combination, which was possibly due to a higher NDF content or lower 3NOP dosage[45]. Co-supplementation of 3NOP with fats or nitrates corresponded with a decreased DMI and milk production, with no further CH4 mitigation[91]. In short, the combination of 3NOP with other additives could enhance the CH4 reduction, but the outcomes are quite variable and largely depend on the type of additive.
Low-efficacy scenarios
-
In most of the experimental studies, 3NOP significantly reduces the CH4 emissions; however, several conditions have been reported in which its mitigation potential was relatively lower. Among the potential determinants, diet composition appears to be the most influential factor. Diets characterized by high NDF and low starch tend to display diminished responses due to the enhanced fiber fermentation, which increases H2 availability for methanogenesis, and offsets 3NOP efficacy[67,113]. In contrast, starch-rich diets stimulate the generation of propionate and reduce rumen pH, which tends to enhance the effectiveness of the inhibitor[114]. Consequently, diets with high NDF, fat, or urea content can inhibit the overall CH4 reduction capacity of the additive[116]. Variability in 3NOP efficacy is also caused by dose-related effects and response plateauing. CH4 mitigation does not increase indefinitely with increasing 3NOP inclusion levels, and responses may plateau at around 100 mg/kg DMI in dairy, and 150−200 mg/kg DMI in beef cattle[93,113]. Similarly, inadequate dosing may not sustain effective ruminal levels, leading to reduced efficacy. In addition, supplementation strategies that result in irregular or intermittent intake can reduce its mitigation efficacy compared with continuous delivery systems like TMR or frequent dosing, because 3NOP is rapidly metabolized in the rumen[52,53,67]. Other factors like animal-related variation (e.g., species and breed differences, parity, and production stage)[50,67,91], interactions with co-supplemented feed additives[42], and methodological differences in CH4 measurement techniques, such as RCS, SF6, or GF, may also influence the magnitude of reported mitigation[54]. Overall, low-efficacy scenarios of 3NOP supplementation are primarily associated with diet composition, suboptimal dosing strategies, and inconsistent delivery methods, highlighting the importance of optimizing these factors to improve CH4-mitigation outcomes in future research.
-
The impact of 3NOP on DMI is dose-dependent and varies across cattle types. In dairy cows, lower doses (40−60 mg/kg DMI) typically have a negligible effect on the intake[50,85,91]. While transient reductions have been observed in early lactation cows at doses as low as 51 mg/kg DMI, these were generally associated with post-calving intake depression and recovered as lactation progresses[94]. However, supplementation at higher doses (≥ 80 mg/kg DMI) consistently suppressed the DMI across the various basal diets, with reductions being more prominent in multiparous cows[86,90,91]. This dose-dependant effect was further confirmed by a meta-regression analysis, reporting a decline of 0.013 kg/d in DMI for every 1 mg/kg increase in the 3NOP dose above the mean level (77.0 ± 33.17 mg/kg DMI)[61]. In grazing dairy cows, a 10.5% decrease in DMI was noticed at a much higher dose rate (130 mg/kg DMI) as compared to feedlot cattle (80 mg/kg DMI)[55,88]. This effect can be attributed to the high-fiber intake during grazing, which could partially offset the 3NOP-induced reduction in CH4 emission[61]. In contrast, beef cattle exhibit higher tolerance, with doses between 100 and 150 mg/kg DMI, typically showing minimal impact on DMI[52,57,97]. While higher doses (200 mg/kg DMI) were reported to reduce DMI by 7%−9%[103,105]. However, some studies reported a dose adaptation protocol, gradually increasing the dose can prevent intake reduction. A stepwise increase in 3NOP doses from 50−200 mg/kg DMI over a period of 1−9 d in beef cattle prevented DMI suppression[104]. Similarly, another study also reported no reduction in DMI at 200 mg/kg DMI, likely due to prior adaptation to lower doses (150 and 175 mg/kg DMI)[100]. A qualitative assessment of data summarized in Table 3 suggests a modest dose-related response of DMI to 3NOP supplementation. At ≤ 60 mg kg/DMI, studies generally report minimal or non-significant effects, with an average decrease of 3%−5%. In the 60−100 mg kg/DMI dose range, reductions become more consistent, averaging 8%−10%. Finally, at > 100 mg/kg DMI, the response remains highly variable, with observed declines ranging from non-significant to as high as 11%−12%, though the overall trend indicates a moderate decline of 6%−8% in DMI. In summary, 3NOP effects on feed intake are not biologically neutral, although low doses may not always affect DMI. Higher levels of 3NOP consistently suppress DMI, and the magnitude of this response varies with diet, feeding protocol, parity, and lactation stage.
Table 3. Effects of 3NOP supplementation on DMI, production performance, and feed efficiency in ruminants.
Animal Type 3NOP dose (mg/kg DMI) DMI (△%) Milk yield (△%) ADG (△%) Feed efficiency (product/DMI) Ref. Dairy Cow 60 ↓5.7 ns − ↓ [83] Dairy Cow 80 ↓5−6 ↓6.6 − ns [84] Dairy Cow 60, 80 ↓9 ↓5 ↓42 ns [86] Dairy Cow 130 ↓6 ↓6 (T) ns ns [55] Dairy Cow 80 ns ns − ↑ [50] Dairy Cow 60 ns ns ns ns [89] Dairy Cow 80 ↓11 ↓7.2 − − [90] Dairy Cow 80 ↓13.4 ↓11.7 ↓168.9 ↓ [91] Dairy Cow 100 ↓16.6 ↓11.4 − − [92] Dairy Cow 48, 51 ns ↓8.7 ns ns [71] Dairy Cow 60, 80 ↓6.5 ↓4.4 − ns [59] Dairy Cow 130 ns ns ↑171.8 ns [48] Beef Cattle 100 ns − ns ↑ [45] Beef Cattle 100, 150 ns − ↓8(T) ns [97] Beef Cattle 200 ↓1.9 − − − [68] Beef Cattle 100, 125, 150 ↓6.4 − − − [99] Beef Cattle 150, 175, 200 ↓5.4 − ns ↑ [100] Beef Cattle 121 ↓11.6 − ↓10.3 ↑ [96] Beef Cattle 100 ns − ns ↑ [45] Beef Cattle 2.5 g d−1 ns − ↑ − [51] Beef Cattle 125, 200, B:80 ↓7 − ns ↑ [103] Beef Cattle 50, 75, 100, 150, 200 ns − ns ↑ (T) [104] Beef Cattle 100, 200 ↓8 − ↓10.3 (T) ↓ [105] (△%): treatment response over control; DMI: dry matter intake; ADG: average daily gain; ECM: energy-corrected milk. Product = ECM for dairy, ADG for beef; ns: not significant; -: not reported; ↓: decreased; ↑: increased; T: numerical tendency (p > 0.05); B: Bovaer@. Milk yield and energy-corrected yields
-
Supplementation of 3NOP at moderate doses (40 to 60 mg/kg DMI) typically has no significant effect on milk yield and energy-corrected milk (ECM)[89,94]. However, higher doses (≥ 80 mg/kg DMI) can significantly reduce milk yield by 7%−12% and ECM by 5%−9%, with greater reductions observed in multiparous cows[43,86,91,92]. In contrast, dairy cows under grazing conditions did not show a decline in yields of milk and ECM even at higher doses (80−130 mg/kg DMI)[55,88]; however, this response is not universal. The effects of 3NOP on milk yield and ECM are also influenced by the basal diet. A reduction in milk yield has been reported for HC diets, whereas high-fiber diets tend to maintain milk yield[61,71]. Milk yield normally declines from early to late lactation, so reductions observed in late lactation may reflect a production-stage effect[50]. A breed-related effect was observed when a noticeable increase in milk yield and ECM in Holstein Friesian cows was reported, with a tendency for a yield reduction in Brown Swiss cows, although overall effects remained statistically non-significant[85]. In summary, the response of milk yield to 3NOP supplementation is variable and becomes increasingly unfavorable with an increase in the dose levels, particularly in multiparous cows or under certain dietary conditions. Therefore, more research is required for a clear understanding of these production trade-offs, which otherwise can remain a significant challenge.
Milk composition
-
Multiple studies consistently reported an increase in milk fat percentage with 3NOP supplementation at moderate doses (60 mg/kg DMI). The reported increase ranged from 3.7% to 6.5% in fat percentage, and 5% in fat yield[56,90,94]. However, at higher doses (≥ 80 mg/kg DMI), a decline in fat yield is often reported, despite an increase in fat percentage, typically due to a reduction in overall milk yield[86,91]. Dietary differences also affect milk fat content, which is generally higher in grass-based diets than in HC and corn-based diets[71,86]. 3NOP has minimal to no effects on milk protein concentration and milk lactose levels[56,89,93]. However, an increase in milk protein percentage with the high dose (2,500 mg/d) was reported, while milk protein yield remained unchanged[53]. Many studies found an increase in the milk urea nitrogen (MUN) in cows supplemented with 3NOP[55,89,93]. One study observed an increase in somatic cell count, though this may be related to herd health, lactation stage, or management practices rather than a direct effect of 3NOP[50]. Mineral and vitamin profiles also showed changes: calcium and vitamin B12 levels increased, potassium decreased, while phosphorus and magnesium remained unchanged. Additionally, κ-casein levels and micelle structure were unaffected[43]. In short, 3NOP generally increases milk fat percentage; however, higher doses may negatively affect milk and milk fat yields. Other milk components remain largely unaffected, but the frequent rise in MUN suggests that 3NOP may impair N use efficiency.
Milk fatty-acid profile
-
Contrary to earlier findings, recent studies have reported a significant effect of 3NOP on milk fatty acid (FA) profiles[53]. Many studies have reported an increase in the short- and medium-chain FAs with 3NOP supplementation[56,93,94]. This may be due to an increased concentration of butyrate[123]. Similarly, trans FA, including trans-10 18:1, trans-11 18:1, and cis-9, trans-11 conjugated linoleic acid levels declined[56,93,94]. Responses of odd- and branched-chain FA (OBCFA), including iso-C15:0 and anteiso-C17:0, which are markers of fibro-lytic bacterial activity, were inconsistent[93,94]. The influence of 3NOP on certain long-chain FAs in milk was also found to be variable with stage of lactation[94]. 3NOP alters the FA profile of milk; notably, the de novo synthesis of saturated FA increased, while unsaturated and trans FA decreased. These changes could have both positive and negative effects on the nutritional profile of milk and consumer acceptability.
Body weight gain and feed efficiency
-
Most studies in dairy cows did not find any effect of 3NOP supplementation on body weight (BW) and average daily gain (ADG), as summarized in Table 3[45,55,89,103]. However, a dose-dependent decrease in average daily gain (ADG) and final body weight for doses exceeding 80 mg/kg DMI, with no effect at lower doses (< 80 mg/kg DMI) was observed in dairy cows[86]. Moreover, the weight gain in the Holstein Frisian was slightly higher than in the Brown Swiss cows, suggesting a breed-specific effect[89]. Many studies revealed that overall, there were no significant impacts of 3NOP on body weight in beef cattle[52,57,105]. However, supplementation of 3NOP (150 mg/kg DMI) in young calves reduced ADG significantly, showing negative effects of 3NOP on growth performance at early ages[96]. Generally, the effect of 3NOP on body weight gain at low to moderate doses is not significant; however, higher doses can significantly affect ADG, particularly in dairy cattle and in young growing animals.
-
Recent literature has consistently shown that supplementation of 3NOP effectively mitigates CH4 emission in ruminants[67,69]. Its CH4 reduction potential is also much greater than most diet-related approaches, e.g., lipids, nitrates, or tannins. Its effect is reversible upon withdrawal, and there has been no indication of microbial adaptation or loss of efficacy, even in long-term studies[93,117]. Moreover, 3NOP is widely applicable to diverse dietary regimes (forage vs concentrate-based), ruminant species (cattle and sheep), and production systems (intensive vs pasture-based)[76,95]. It can be readily incorporated into current feeding regimens. At recommended dosages, it has minimal to no negative impact on animal performance; some studies even reported enhanced productivity i.e., increased milk fat concentration, improved feed efficiency, and ADG in beef cattle[50,54,65]. The most important benefit of 3NOP over other inhibitors like bromochloromethane, 2-bromoethane sulfonate, seaweeds such as Asparagopsis taxiformis and Asparagopsis armata, is its safety profile. Most of the safety-related studies have reported no evidence of its metabolic residues in blood, milk, or meat, and no associated adverse environmental impacts[33,43,44]. 3NOP specifically inhibits the methanogens without profoundly changing total bacteria, protozoa, and fungi[75,76,81]. It increases fibro-lytic and propionate or butyrate-producing bacterial genera and reduces acetate-producing bacteria[77,124]. This selective microbial modulation allows the rumen ecosystem to maintain overall functionality with reduced CH4 production, and redirects metabolic H2 towards propionate or butyrate instead of acetate[55,93]. Similarly, a reduction in NH3-N with 3NOP suggests more efficient dietary nitrogen utilization[57,71].
Challenges
-
The dependency of 3NOP efficacy on different factors remains a major challenge. Its efficacy is constantly decreased in diets with NDF content or in fat- and urea-based diets. Similarly, increasing the 3NOP dose enhances mitigation up to a threshold but efficacy becomes plateaued beyond a certain point, and further dose escalation offers no additional benefit while potentially impairing animal performance. Efficacy also reduces when delivery mechanisms are not effective in maintaining constant intake, or supplementation time is not aligned with peak CH4 production. Further variability arises from species- and breed-specific differences[53,67,69,116], which pose significant challenges for its practical application. Similarly, in pasture-based systems, the efficacy of 3NOP is limited due to difficulty in its continuous supply and less rumen residence time[55,88]. For making the 3NOP evenly effective in grazing animals, the development of effective slow-release or water-based delivery systems are still undergoing investigations[106]. Supplementation of 3NOP at higher doses is often implicated with negative effects on animal performance, including a decrease in DMI, milk yield, and ADG[86,93]. Therefore, identifying optimal dose ranges to get maximum efficacy without affecting animal performance remains a challenge. Being a synthetic feed additive, 3NOP's safety profile and consumer acceptance also remain a key concern. Although it is approved for use by many regulatory agencies and countries, limited available long-term safety studies, recently reported health issues in Danish dairy cows, and the absence of approval in major livestock-producing countries such as India and China reflect persistent uncertainty regarding its safety. Many short- and long-term trials conducted till now have reported no microbial adaptation, but there is still a need for large-scale and multi-season field studies to confirm its impacts on the rumen microbiome, nutrient utilization, and environmental footprint under practical farming conditions[49,76]. The inclusion of 3NOP can raise feed costs, potentially discouraging its adoption without a policy or carbon-credit incentives[125]. A major non-technical challenge is public preference for natural over synthetic compounds like 3NOP, makes its acceptance limited.
-
Optimizing the dose and delivery of 3NOP is critical for maximizing its efficacy while minimizing potential side effects and economic costs. The goal of precision dosing strategies is to tailor 3NOP inclusion rates to animal-specific factors, management protocols, and dietary composition to prevent under- or over-supplementation[104]. Implementing this concept requires a predictive algorithm that integrates biological and nutritional variables. Key inputs should include animal-specific factors (e.g., species, breed, BW, DMI, physiological stage, parity, and baseline CH4 yield) and diet-specific variables (e.g., NDF and starch concentrations, forage-to-concentrate ratio). Furthermore, management-related parameters such as feeding frequency, delivery method (e.g., top-dress, premix, or water-based systems[106]), and adaptation duration must be accounted for. Within this framework, the algorithm would predict the optimal inclusion rate (mg/kg DMI), the expected CH4 reduction, and potential impacts on DMI and emission intensity. Such models could be developed using regression-based meta-analysis or machine learning techniques trained on robust, multi-study datasets. Additionally, 3NOP might be incorporated into precision livestock farming technologies, including automated feeders, wearable, and real-time monitoring devices to improve the accuracy of dosing and provide opportunities to adjust it in response to the physiological state and behavior of animals.
Diet-, host-, and system-specific optimization of 3NOP efficacy
-
The effectiveness of 3NOP under various diet compositions (NDF, starch, fat, and protein levels), production systems (feedlot vs pasture), and animal-related factors (species, breed, production stage, and parity) can be assessed by large-scale studies. These findings will serve to further refine the models discussed earlier, allowing for more precise, data-driven guidance on optimal dosage strategies. Further studies are also required to focus on synergistic interactions between 3NOP and other mitigation agents, such as dietary lipids, tannins, nitrates, essential oils, and ionophores to enhance CH4 mitigation, without adverse impacts on the production efficiency of animals.
Long-term microbiome programming
-
It has been demonstrated that early-age 3NOP supplementation in calves can cause long-term rumen microbiome shifts, which result in the continued reduction of CH4 emissions even after the withdrawal[82]. Based on these observations, we hypothesize that the 3NOP supplementation during the critical window of early-life rumen colonization, when the microbial ecosystem is unstable and highly responsive to external interventions, can permanently alter the trajectory of microbial assembly, leading to a persistently lower methanogenic capacity. Application of 3NOP at this early colonization stage may selectively inhibit methanogenic archaea, thereby promoting the establishment of alternative H2-utilizing pathways and ultimately result in a more stable, low-methanogenic rumen ecosystem in the future. However, long-term studies are not only needed to validate these initial findings, but also to determine its optimal timing, dosage, route of delivery, microbial, and metabolic mechanisms involved[76].
Understanding the Fate of Spared H2
-
Methane mitigation spares the H2, which is typically redirected toward alternative metabolic pathways, e.g., propionate formation. However, a further detailed understanding is required to have a better understanding and accurate measurement of this redirected flow under different dietary conditions. These understandings would allow strategic control of rumen fermentation to favor even more desirable end-products, and improve overall production efficiency[58].
Socio-economic and environmental evaluation of sustainable adoption
-
The holistic evaluation of the environmental and socio-economic impacts of 3NOP is a prerequisite to its sustainable adoption as an anti-methanogenic feed additive. Future life-cycle assessment research needs to measure important environmental indicators such as enteric CH4 intensity (g CH4/kg product), carbon footprint (kg CO2-eq/unit product), manure-derived CH4 and N2O emissions, and feed efficiency-adjusted greenhouse gas outputs. These assessments must consider the variations in DMI, productivity, nutrient excretion, and upstream emission to calculate net system-level benefits. From a policy perspective, integrating 3NOP into carbon credit schemes, greenhouse gas offset programs, subsidy frameworks, and sustainable livestock certification will facilitate its adaptation and help in transitioning from controlled experimental settings to widespread, real-world implementation.
Alternative and next-generation methane inhibitors
-
Based on the success of 3NOP, future studies need to identify structural analogs of the MCR enzyme. These next-generation inhibitors may offer improved binding affinity, stability, and persistence in the rumen, leading to enhanced inhibition efficiency. Potential candidates include naturally derived compounds such as phytochemicals and biosynthesized inhibitors. Such innovations could expand the toolbox for enteric CH4 mitigation in diverse livestock systems.
Long-term safety and chronic exposure assessment
-
Most of the studies are short-term (8−12 weeks) and provide little insight into long-term exposure, multi-lactation effects, or potential adaptive responses of methanogens. Prolonged impacts on liver function, immunity, systemic nitrate load, and reproduction also remain largely unknown. Furthermore, research on the metabolism, fate of 3NOP and its metabolites in ruminants is also very limited. Therefore, long-term, multi-lactation studies are required to build regulatory confidence.
Stability and on-farm delivery losses of 3NOP
-
The stability and delivery losses of 3NOP is the least-studied area, and systematic investigations are required to quantify its degradation during premix storage, and exposures to humidity, trace minerals, and heat during pelleting and feed processing. Similarly, its stability in silage, concentrate pellets, and TMR stored for extended periods remains largely unknown. Future research should systematically investigate 3NOP losses under diverse storage, processing, and feeding conditions, so its efficacy can be predicted accurately.
-
3NOP stands out as one of the most effective feed additives for enteric CH4 mitigation, achieving reductions of 21%−87.6% (g/kg DMI) across ruminant species through selective inhibition of methyl-coenzyme M reductase without substantially disrupting rumen fermentation, and has less impact on nutrient utilization or animal performance at recommended doses.
However, its mitigation responses are highly variable, with reductions below 20% reported under certain conditions. Such variability is primarily governed by dosage, diet composition, and delivery method, with consistently lower efficacy under high-fiber and grazing systems. Moreover, it has potential trade-offs in intake and productivity at higher inclusion rates. Addressing these challenges, together with cost, safety, and regulatory constraints, through slow-release formulations, precision dosing, diet- and system-specific optimization, coupled with comprehensive safety assessments, will position 3NOP as a scalable and practical tool for rapid CH4 abatement and sustainable livestock production.
This study was supported by the Agricultural Science and Technology Innovation Program (No. CAAS-IFR-ZDRW202302) and Beijing Livestock Innovation Consortium (BAIC05).
-
Not applicable.
-
The authors confirm their contributions to this study as follows: Zeeshan M conducted the literature search, compiled and synthesized the relevant studies, and drafted the manuscript. Liu Y and Zhang X contributed to the conception and overall design of the work. Khan NA and Tu Y critically revised the manuscript for important intellectual content. All authors reviewed and approved the final version of the manuscript.
-
All data and information discussed are derived from previously published literature, which has been appropriately cited within the manuscript. No new datasets were created or analyzed during the preparation of this article.
-
The authors declare that they have no conflict of interest.
- Copyright: © 2026 by the author(s). Published by Maximum Academic Press, Fayetteville, GA. This article is an open access article distributed under Creative Commons Attribution License (CC BY 4.0), visit https://creativecommons.org/licenses/by/4.0/.
-
About this article
Cite this article
Zeeshan M, Khan NA, Zhang X, Liu Y, Tu Y. 2026. 3-Nitrooxypropanol as a rumen methane mitigation agent: mechanisms, efficacy, and future directions. Circular Agricultural Systems 6: e022 doi: 10.48130/cas-0026-0017 
3-Nitrooxypropanol as a rumen methane mitigation agent: mechanisms, efficacy, and future directions
- Received: 26 January 2026
- Revised: 24 March 2026
- Accepted: 21 April 2026
- Published online: 08 September 2026
Abstract: Enteric methane (CH4) accounts for approximately 17% of global anthropogenic greenhouse gas emissions and the loss of 2%−12% of feed energy in ruminants. To mitigate its adverse effects on global warming and animal production, efforts have been directed towards developing cost-effective and eco-friendly mitigation strategies. Among these, 3-nitrooxypropanol (3NOP) has emerged as one of the most effective mitigating compounds. This review summarizes the mechanism of action, key modulatory factors, safety considerations, production implications, and future prospects of 3NOP. 3NOP mitigates methanogenesis by selectively inhibiting the methyl-coenzyme M reductase without disrupting the rumen fermentation. 3NOP reduces CH4 yield, with reported reductions of 21%−59.5% in dairy and 22%−87.6% in beef cattle. However, mitigation responses are highly variable, and reductions below 20% have also been reported. This variability is influenced by factors such as dosage, diet composition, delivery method, production stage, and ruminant species, with consistently lower responses being observed under high-fiber and pasture-based diets. Despite its targeted mechanism, 3NOP is not biologically neutral, and at higher inclusion rates it can depress dry matter intake and milk yield in dairy cows, indicating production trade-offs. 3NOP is considered safe; however, limited long-term studies across diverse production systems, and pending regulatory approvals in major livestock-producing countries like China, are highlighting the need for further safety evaluation. Future research should address key challenges, including dose optimization, delivery methods, dietary dependencies, production impacts, and reduced efficacy under grazing conditions. Additionally, comprehensive life-cycle analyses and socio-economic assessments are essential for its widespread adoption.