











-
Cucumber (Cucumis sativus L., 2n = 2x = 14) is an annual creeping or climbing herbaceous plant belonging to the genus Cucumis within the Cucurbitaceae family. It is believed to have originated in the South Asian foothills of the Himalayas approximately 3,000 years ago, a region characterized by abundant light resources[1]. Cucumber has become one of the most widely cultivated vegetable crops worldwide. According to FAOSTAT, the global cucumber cultivation area exceeded 2.28 million hectares in 2024, with total production reaching more than 87.84 million tons.
Given its global agricultural importance, improving cucumber yield and quality has become a major research focus. Among the traits affecting crop performance, leaf color represents a critical phenotypic indicator closely associated with plant growth and physiological status. Leaf color largely reflects chlorophyll content and photosynthetic efficiency. Healthy green leaves support efficient photosynthesis, providing the energy and nutrients required for fruit development. In contrast, abnormal leaf coloration—such as chlorosis or lesion formation—can reduce photosynthetic capacity and ultimately affect fruit growth and yield.
Beyond its role in photosynthesis, leaf color also serves as a sensitive indicator of plant physiological and nutritional status. For example, nitrogen deficiency typically causes progressive chlorosis beginning from older leaves[2]. Therefore, understanding the genetic regulation of leaf color offers a direct route to enhancing photosynthetic capacity for boosting global yield stability, as well as providing an effective approach for assessing plant health, nutrient balance, and disease resistance in cucumber for optimizing cultivation practices.
Leaf color in plants is determined by the composition and concentration of several pigments, including chlorophyll, carotenoids, lutein, and anthocyanins. Under normal growth conditions, the relatively high abundance of chlorophyll gives leaves their typical green coloration. Alterations in pigment composition or concentration, caused by genetic mutations or environmental factors, can lead to various leaf color phenotypes. In cucumber, the common type of leaf color mutation is the virescent phenotype, in which young leaves initially appear yellow and gradually turn green as the seedlings grow[3−9]. In contrast, variegated or mottled leaf mutants are relatively rare, with only one reported case[10]. In addition, five albino mutants were reported[11−14], while other mutants display varying degrees of yellow-green coloration (Fig. 1). Although these phenotypic categories provide a useful framework, they do not directly reflect the underlying molecular mechanisms, which are often shared across different visual classes.
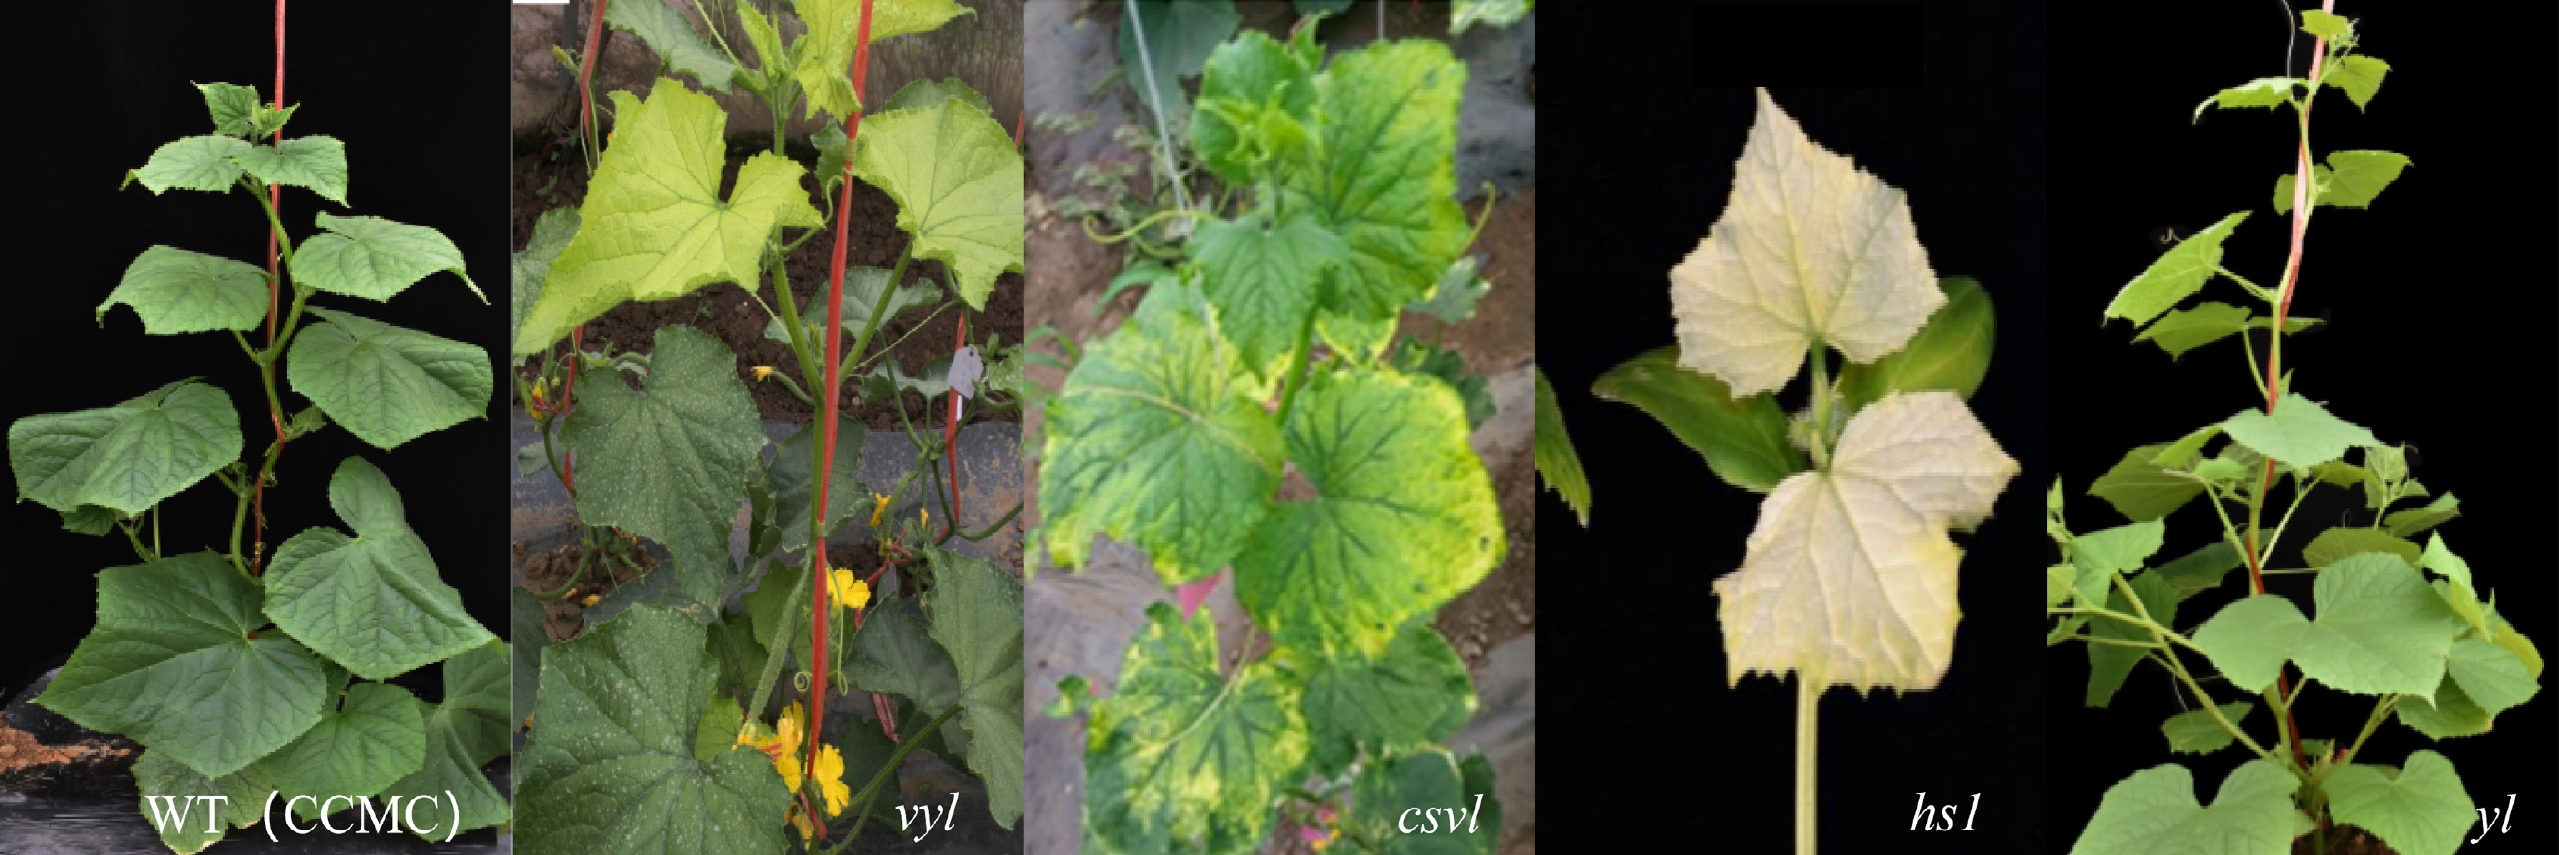
Figure 1.
Phenotypic comparison of cucumber leaf color mutants. The wild type ('WT', CCMC) and four cucumber seedlings with typical leaf color variations, vyl, csvl, hs1, and yl, are shown from left to right. The WT (CCMC) displays normal green leaves. Among them, vyl showed that the young leaves turned green gradually with growth; csvl showed mottled yellow and green; hs1 showed that the leaves of the plant were albino; yl showed the yellow phenotype.
In recent years, substantial progress has been made in elucidating the genetic basis and molecular mechanisms underlying leaf color variation in cucumber. This review synthesizes current advances in the identification and functional characterization of leaf color-related genes in cucumber. We highlight the mapped key genes involved in pigment-biosynthesis pathways and chloroplast development, discuss their regulatory mechanisms and pleiotropic effects, and outline future research aspects (Supplementary Table S1). In addition, we discuss the potential application of leaf-color mutations as visible marker traits in haploid induction, hybrid breeding, and cucumber cultivar improvement.
-
Leaf color mutations in cucumber originate from spontaneous mutation and artificial mutagenesis, which together constitute the primary genetic resources for mapping and functional studies. Spontaneous mutations arise naturally under environmental influences such as light, temperature, and soil, and usually manifest as single-gene variations. Although their occurrence is relatively rare, the distinct visual phenotypes make them readily identifiable and valuable for genetic analysis and breeding, as exemplified by mutants such as v-1, v-2, v-3, and ygl1[4,6,15,16].
In contrast, artificial mutagenesis is currently the most widely used approach for producing vegetable leaf-colored mutants in cucumbers and other vegetable crops. Various techniques have been employed, including chemical induction (e.g., EMS), physical induction (e.g., gamma rays), and insertional mutagenesis (e.g., T-DNA or transposon insertion)[17]. For example, the golden-yellow leaf mutant gl, yellow leaf yl and yl-2 were generated through EMS induction, while yellowing mutants yl-5 and tnyl-2 were obtained via Tnt1 retrotransposon insertion[13,18−21]. These approaches have greatly accelerated the identification of leaf color-related loci in cucumber.
In total, 24 leaf color loci have been reported in cucumber, spread across six of the seven chromosomes (Fig. 2). They all have single-gene inheritance. Among them, 83% are identified as recessive traits, and 79% have been proposed for candidate genes. These leaf color phenotypes represent the macroscopic reflection of alterations in chloroplast structure and pigment metabolism pathways. In many cucumber leaf color mutants, photosynthetic pigment content is significantly reduced, accompanied by abnormalities in chloroplast ultrastructure, such as disrupted grana stacking and decreased starch grain accumulation. These structural defects are often associated with reduced photosynthetic parameters, including net photosynthetic rate and stomatal conductance. Together, these physiological and cellular abnormalities indicate that cucumber leaf color mutations are typically caused by disruptions in specific molecular regulatory pathways, which can be broadly categorized into three aspects: chloroplast development, pigment metabolic network, and nuclear-cytoplasmic interactions (Supplementary Table S1).
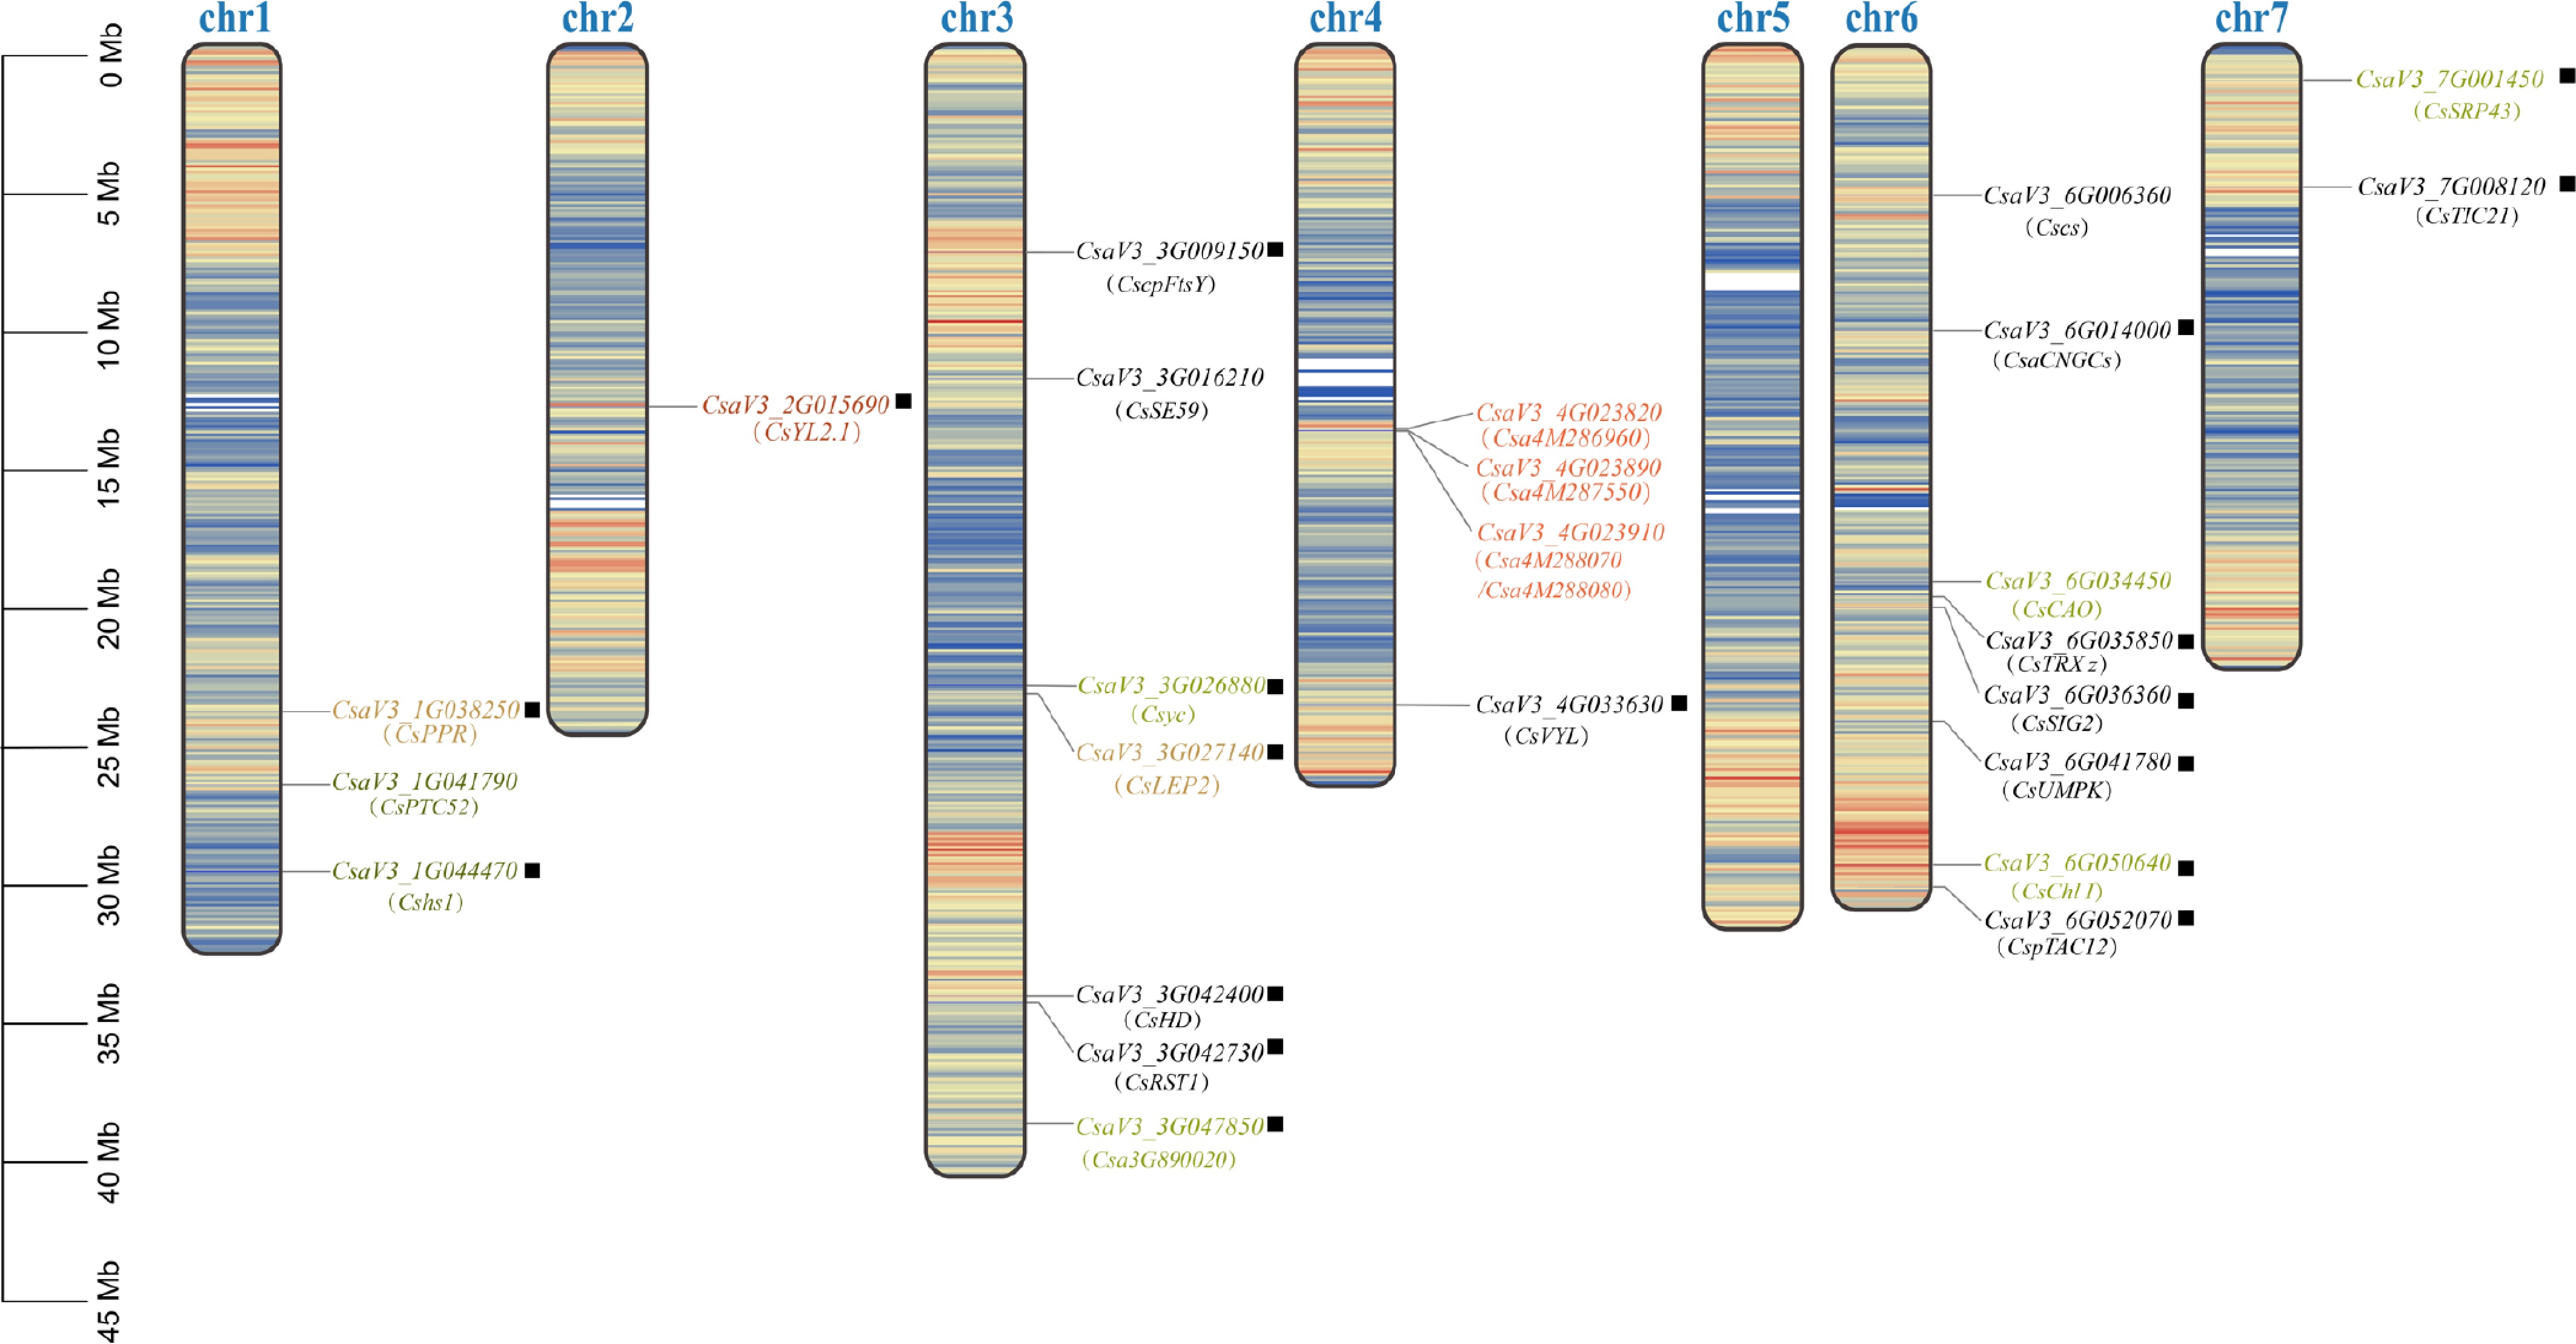
Figure 2.
The distribution of candidate genes identified for leaf color in cucumber (Cucumis sativus). The gene ID was noted in reference genome 9930 v3.0. The blue to red color in the chromosome represents that the density of genes on the chromosome is from low to high within 100 kb windows. The gene IDs are color-coded based on the molecular mechanisms they regulate: green for the chlorophyll metabolic pathway, yellow for the nuclear-cytoplasmic interaction pathway, orange for the carotenoid metabolic pathway, and black for the chloroplast biogenesis pathway. Black squares denote genes that have been fine-mapped.
-
Chloroplasts are specialized plastids that drive photosynthesis and support a wide range of essential metabolic processes in plants, including the biosynthesis of amino acids, fatty acids, nucleotides, pigments, and phytohormones. Chloroplast biogenesis starts with the formation of proplastids, as well as regulates chlorophyll synthesis and thylakoid formation[22]. In cucumber, 12 out of 24 leaf color mutants arise from the chloroplast biogenesis and structural maintenance of chloroplasts (Supplementary Table S1). Among these, three genes—CsUMPK, CsTIC21, and CsFtsH—are associated with albino phenotypes, causing complete chloroplast defects and seedling lethality[12−14], while the rest lead to varying levels of yellow-green, revealing a diverse set of genes in different aspects of chloroplast biogenesis. These aspects include: 1) protein targeting and import into chloroplasts; 2) protein folding and proteostasis; and 3) metabolic and nucleotide support for plastid development (Fig. 3).
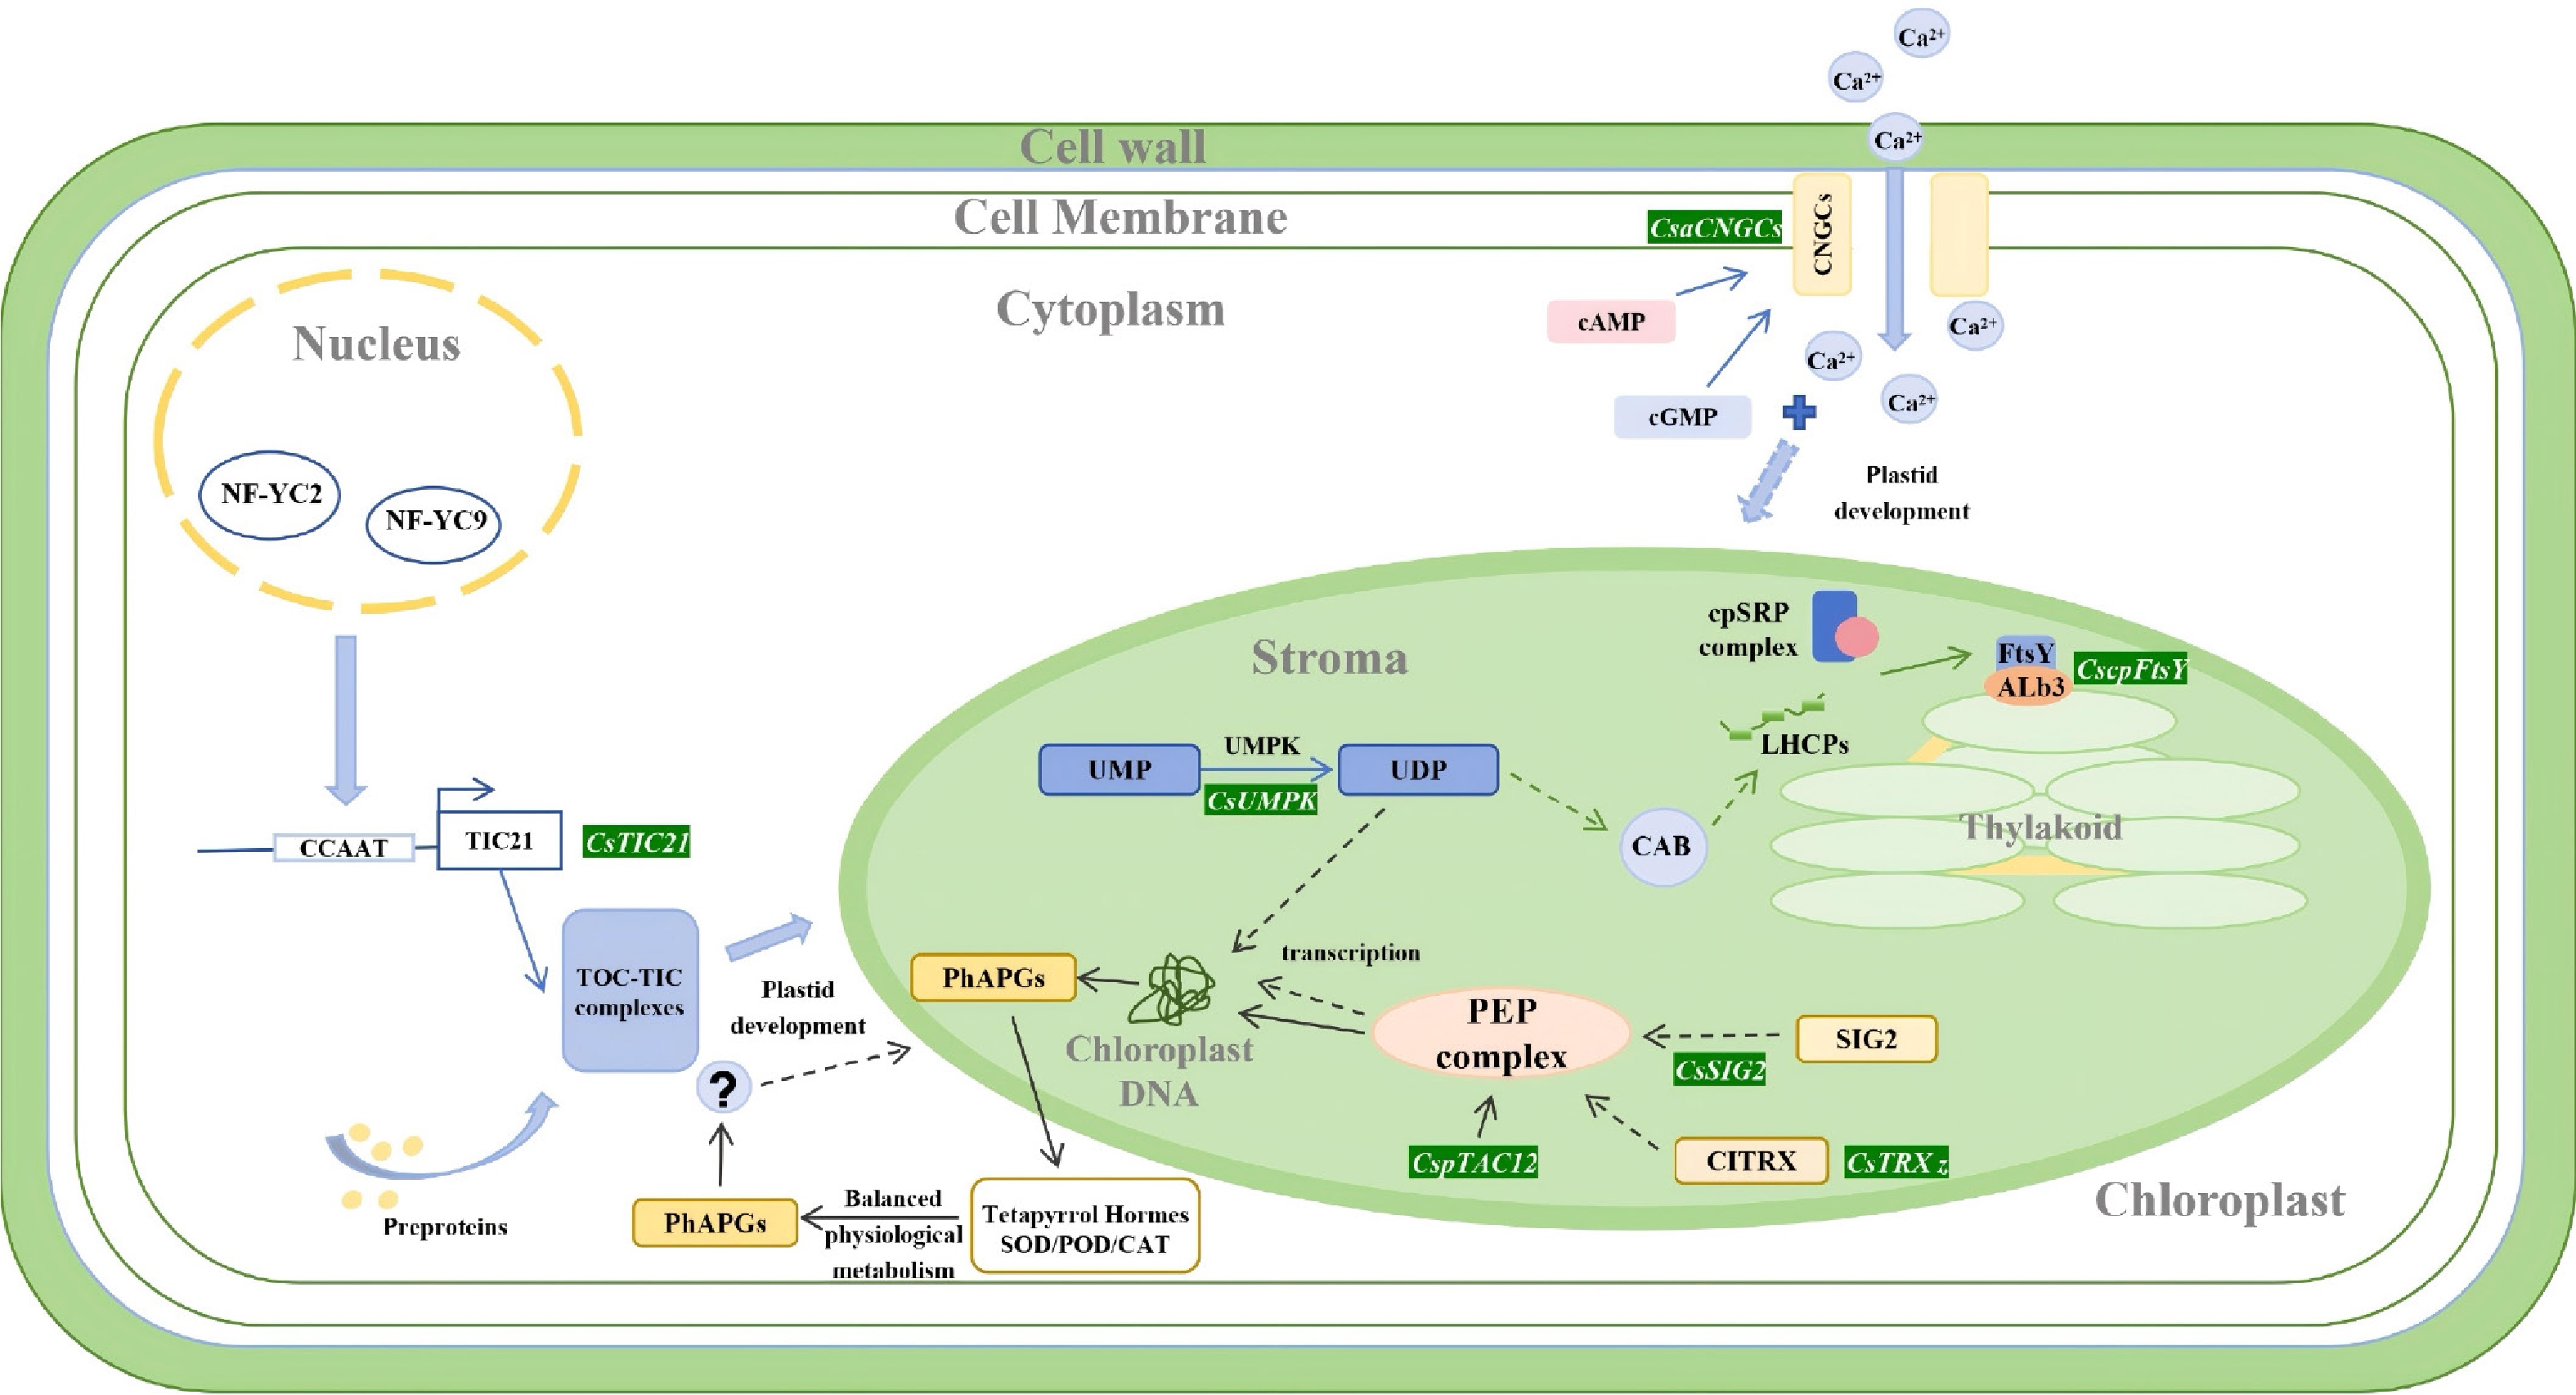
Figure 3.
Schematic model of the molecular network regulating chloroplast biogenesis and maintenance. Chloroplast development requires the precise coordination of nuclear-encoded factors, plastid transcription, structural assembly, and metabolic support. Protein Import and Thylakoid Targeting: Nuclear transcription factors (e.g., NF-YC2/9) activate the expression of CsTIC21, a core component of the TOC-TIC complex, ensuring the import of cytoplasm-synthesized preproteins. Concurrently, CscpFtsY functions in the cpSRP pathway to facilitate the insertion of light-harvesting chlorophyll-binding proteins (LHCPs) into the thylakoid membrane. Plastid Transcription: The expression of chloroplast DNA is heavily dependent on the plastid-encoded RNA polymerase (PEP) complex. This complex is structurally stabilized by CsTRXz (CITRX) and recruited to specific targets by sigma factors such as SIG2. Metabolic and Ion Signaling Support: Enzymatic conversion of UMP to UDP by UMP provides essential nucleotide precursors for thylakoid formation. Additionally, cell membrane-localized CsaCNGCs mediate cAMP/cGMP-dependent influx, triggering signaling for plastid development. Genes highlighted in a green background (e.g., CsTIC21, CscpFtsY) represent the key regulatory genes identified in cucumber.
The majority of chloroplast proteins (> 90%) are encoded by the nucleus, translated in the cytosol, and imported post-translationally via N-terminal transit peptides[23]. This active process requires energy (ATP/GTP) and occurs through the TIC/TOC translocon complex or the chloroplast signal recognition particle (cpSRP) pathway. In cucumber, disruption of CsTIC21, a core component of the translocon at the inner chloroplast membrane, leads to albino cotyledons and seedling lethality, due to a complete failure in protein import and chloroplast differentiation[12]. Two nuclear transcription factors, CsNF-YC2 and CsNF-YC9, directly bind to the CsTIC21 promoter and activate its expression during early seedling development. This regulatory module integrates light signaling and developmental cues to coordinate the onset of chloroplast protein import capacity[12]. Similarly, CscpFtsY, encoding the receptor of the chloroplast signal recognition particle (cpSRP) complex, is essential for the insertion of light-harvesting chlorophyll-binding proteins into the thylakoid membrane; its mutation results in yellow leaves with disorganized thylakoid stacks[21]. It has been proposed that cpFtsY is assembled to the thylakoid membrane and is required for light-harvesting chlorophyll protein (LHCPs) insertion into the membrane[24]. Nymark et al. also reported that cpFtsY could trigger the induction of proteins involved in chloroplastic Fe–S cluster formation in diatoms/green algae that is different from plants[25]. Another virescent leaf mutant v-3, was proposed to be regulated by the CsRST1 gene (RNA exosome supercomplex subunit Resurrection1), which might interrupt chloroplast development via regulating plastid division2 (PDV2)[7]. However, this candidate mutant gene was identified from a pool of 106 genes within a relatively broad 1.34-Mb genomic interval. Due to the lack of fine mapping, its presumed function remains largely speculative. In addition, the existing literature for homologs in other species does not provide a strong association between the gene and the leaf color phenotype, which needs further verification[26−28].
Beyond protein import, chloroplast development relies on robust protein folding, assembly, and degradation systems to maintain proteostasis. Chloroplast proteostasis is maintained by the chloroplast protein quality control (cpPQC) system[29]. At its core, the ATP-dependent chaperone cpHSP70-1 coordinates with co-chaperones like CGE and J-proteins (e.g., DnaJ homologs) to enhance substrate binding. Together, this network mediates protein folding, assembly, translocation, and degradation[30]. In cucumber, a mutation in CsVYL, which encodes a DnaJ-like finger protein, may lead to a change in the domain of the DnaJ-like zinc finger protein, reducing its chaperone binding efficiency[5]. The resulting defective protein folding and delayed thylakoid assembly lead to impaired photosynthetic complexes and a virescent yellow phenotype in young leaves, which subsequently recover their green color[5]. In addition, a cluster of CsFtsH (CsaV3_6G046620 and CsaV3_6G046630), which encodes the FtsH (FILAMENTOUS TEMPERATURE-SENSITIVE H) protease, was proposed to be responsible for the albino phenotypes of alc in cucumber[14]. The double mutants ftsh1ftsh5 and ftsh2ftsh8 in Arabidopsis thaliana also have an albino-like phenotype[31,32]. Studies have shown that FtsH plays an indispensable role in both biogenesis and maintenance of thylakoid membranes during chloroplast development, as well as participating in the degradation of the core components of photosystem II (PSII)[33]. Although CsFtsH seems to be the best candidate for the alc mutant, the causal genotypic variants leading to albino phenotypes were still lacking[14]. Furthermore, Zhou et al. reported a Dominant Virescent Leaf (DVL) phenotype in cucumber, which displays transient yellow-green cotyledons and first true leaf under low temperature conditions that later recover to green under a normal temperature environment[9]. Its causal gene was identified as CsTRXz, which encodes a z-type thioredoxin protein. Thioredoxin (Trx), with seven distinct subtypes (f-, m-, x-, y-, z-, o-, and h-), is a small protein that is mainly responsible for the thiol/disulfide-based redox regulation[34]. TRX z binds to the fructokinase-like proteins FLN1 and FLN2, which are essential components of the plastid transcriptionally active chromosome (pTAC) and the plastid-encoded RNA polymerase (PEP)[35,36,37]. The rice white panicle 2 mutant was caused by a mutation in OsTRX z, which displayed temperature-sensitive phenotypes as well[37]. OsTRX z protein could physically interact with plastid multiple organellar RNA editing factors (MORFs), involved in chloroplast RNA editing that is especially required at high temperature[37]. Another cucumber v-1 mutant initially develops light yellow cotyledons and early leaves that progressively green upon full expansion. This virescent phenotype is driven by mutations in CsCNGCs, which disrupt essential CNGC-mediated Ca2+ influx and cGMP/Ca2+ signaling, ultimately causing chloroplast developmental defects and early etiolation[4].
Proper chloroplast function also imposes substantial metabolic demands, including the need for nucleotide synthesis, energy supply, and precursor metabolites. The characterization of the tnyl2 mutant, generated by Tnt1 retrotransposon insertion, revealed that loss of CsUMPK function leads to stunted growth, photobleached leaves, and severely impaired chloroplast ultrastructure[13]. CsUMPK encodes a uridine monophosphate (UMP) kinase that phosphorylates UMP to form uridine diphosphate (UDP), which is a key enzyme in the pyrimidine metabolic pathway responsible for nucleotide interconversion as building blocks for nucleic acids and central metabolites[38]. Although experimental localization of CsUMPK has yet to be performed, bioinformatic prediction using[13]. Cell-PLoc 2.0 suggests a chloroplast localization. Its orthologs in rice (ygl8/yl2) and Arabidopsis (PUMPKIN/DPT1) are chloroplast-localized, and exhibit similar albino or pale-green phenotypes when mutated, with defects in thylakoid development and chloroplast ATPase (cpATPase) activity[39−42]. Transmission electron microscopy of cucumber tnyl2 showed disrupted thylakoid membranes and a paucity of stacked grana, correlating with a near-complete loss of chlorophyll and compromised PSII activity[13].
Beyond nucleotide metabolism, chloroplast development also relies on the proper functioning of primary metabolic pathways that supply essential biosynthetic intermediates. One prominent example is the shikimate pathway, which channels up to 30% of photosynthetically fixed carbon to produce diverse essential compounds, including aromatic amino acids, pigments, hormones, and antioxidants[43]. These metabolites are vital for chloroplast redox balance and photoprotection, where chorismate synthase is the terminal enzyme that catalyzes chorismate biosynthesis. A mutation in the Cscs gene, which encodes chorismate synthase, is responsible for the persistent leaf-mottling phenotype observed in the cucumber csvl mutant with a green-yellow-white variegation phenotype[10]. The impaired chorismate synthesis disrupts the production of those vital metabolites, leading to photooxidative damage, reduced chlorophyll content, and increased oxidative enzyme activity[10].
In addition to metabolic supply, enzymatic regulators also play important roles in chloroplast development. Most known HD-domain proteins function as phosphohydrolases and have been implicated in this process[44]. In cucumber, CsHD encodes a putative histidine-aspartic (HD) domain-containing protein that was identified as the causal gene for an EMS-induced mutant ‘C777’ characterized by yellow cotyledons and newly emerged true leaves with persistent green dots that gradually regreen during development[45]. Consistent with this, mutations in rice HD-domain genes lead to altered leaf coloration, abnormal chloroplast development, and reduced chlorophyll content[46,47]. Nevertheless, the precise mechanisms by which HD-domain proteins regulate chloroplast development and chlorophyll synthesis remain to be elucidated.
At the transcriptional level, proper chloroplast development further depends on the coordinated expression of plastid-encoded genes. Liu et al. demonstrated that mutant Csvl-6 resulted from an amino acid substitution in CsSIG2, a sigma factor associated with the PEP, impairing chloroplast gene transcription, severely delaying thylakoid development, and reducing chlorophyll synthesis at the seedling stage, which results in a transient yellowing of cotyledons and new leaves that gradually regreen[3]. In Arabidopsis, SIG2 functions as a subunit of PEP to regulate chloroplast development and chlorophyll biosynthesis[48]. Mechanistically, SIG2 exerts a 'dual impact' on transcription: it directly and non-redundantly recruits PEP to specific targets (e.g., tRNA genes trnE, trnY, trnD, and trnV1), while its absence also triggers a moderate, genome-wide reduction in PEP binding[49]. Consistent with this regulatory framework, CspTAC12, a core nuclear-encoded component of the PEP complex, is found essential for chloroplast development[50]. A spontaneous mutation in CspTAC12 results in an albino lethal phenotype, which could be rescued via grafting[50]. Further transcriptomic and physiological analyses revealed that the loss of CspTAC12 function leads to a collapse of PEP-dependent transcription, thereby triggering a broad retrograde signaling response from chloroplast to nucleus.
Broader metabolic regulatory networks may also indirectly influence chloroplast development. The INV/PMEI (invertase/pectin methylesterase inhibitor) superfamily functions as a central hub linking carbohydrate metabolism and cell wall dynamics by post-translationally regulating INV and PME activities[51]. Through the modulation of sucrose partitioning and pectin methylesterification, these proteins exert widespread impacts on plant morphogenesis, organogenesis, and yield traits[52]. Building on these roles, Zhou et al. hypothesized that INV/PMEIs may also participate in regulating chloroplast development and chlorophyll biosynthesis[8]. It might be responsible for a virescent mutant that has normal cotyledons and light green true leaves at the early growth stage that turn green later. However, the underlying molecular mechanisms remain to be elucidated[8].
Integrated pigment biosynthesis and metabolic network: chlorophyll, carotenoid, and heme pathways
Tetrapyrrole metabolism and chlorophyll dynamics
-
Chlorophyll and heme share a common tetrapyrrole biosynthetic pathway, making the regulation of metabolic flux at key branch points critical for pigment homeostasis. Chlorophyll synthesis starts from L-glutamyl-tRNA to chlorophyll a, and then to chlorophyll b. The process is mainly summarized into four steps (Fig. 4).
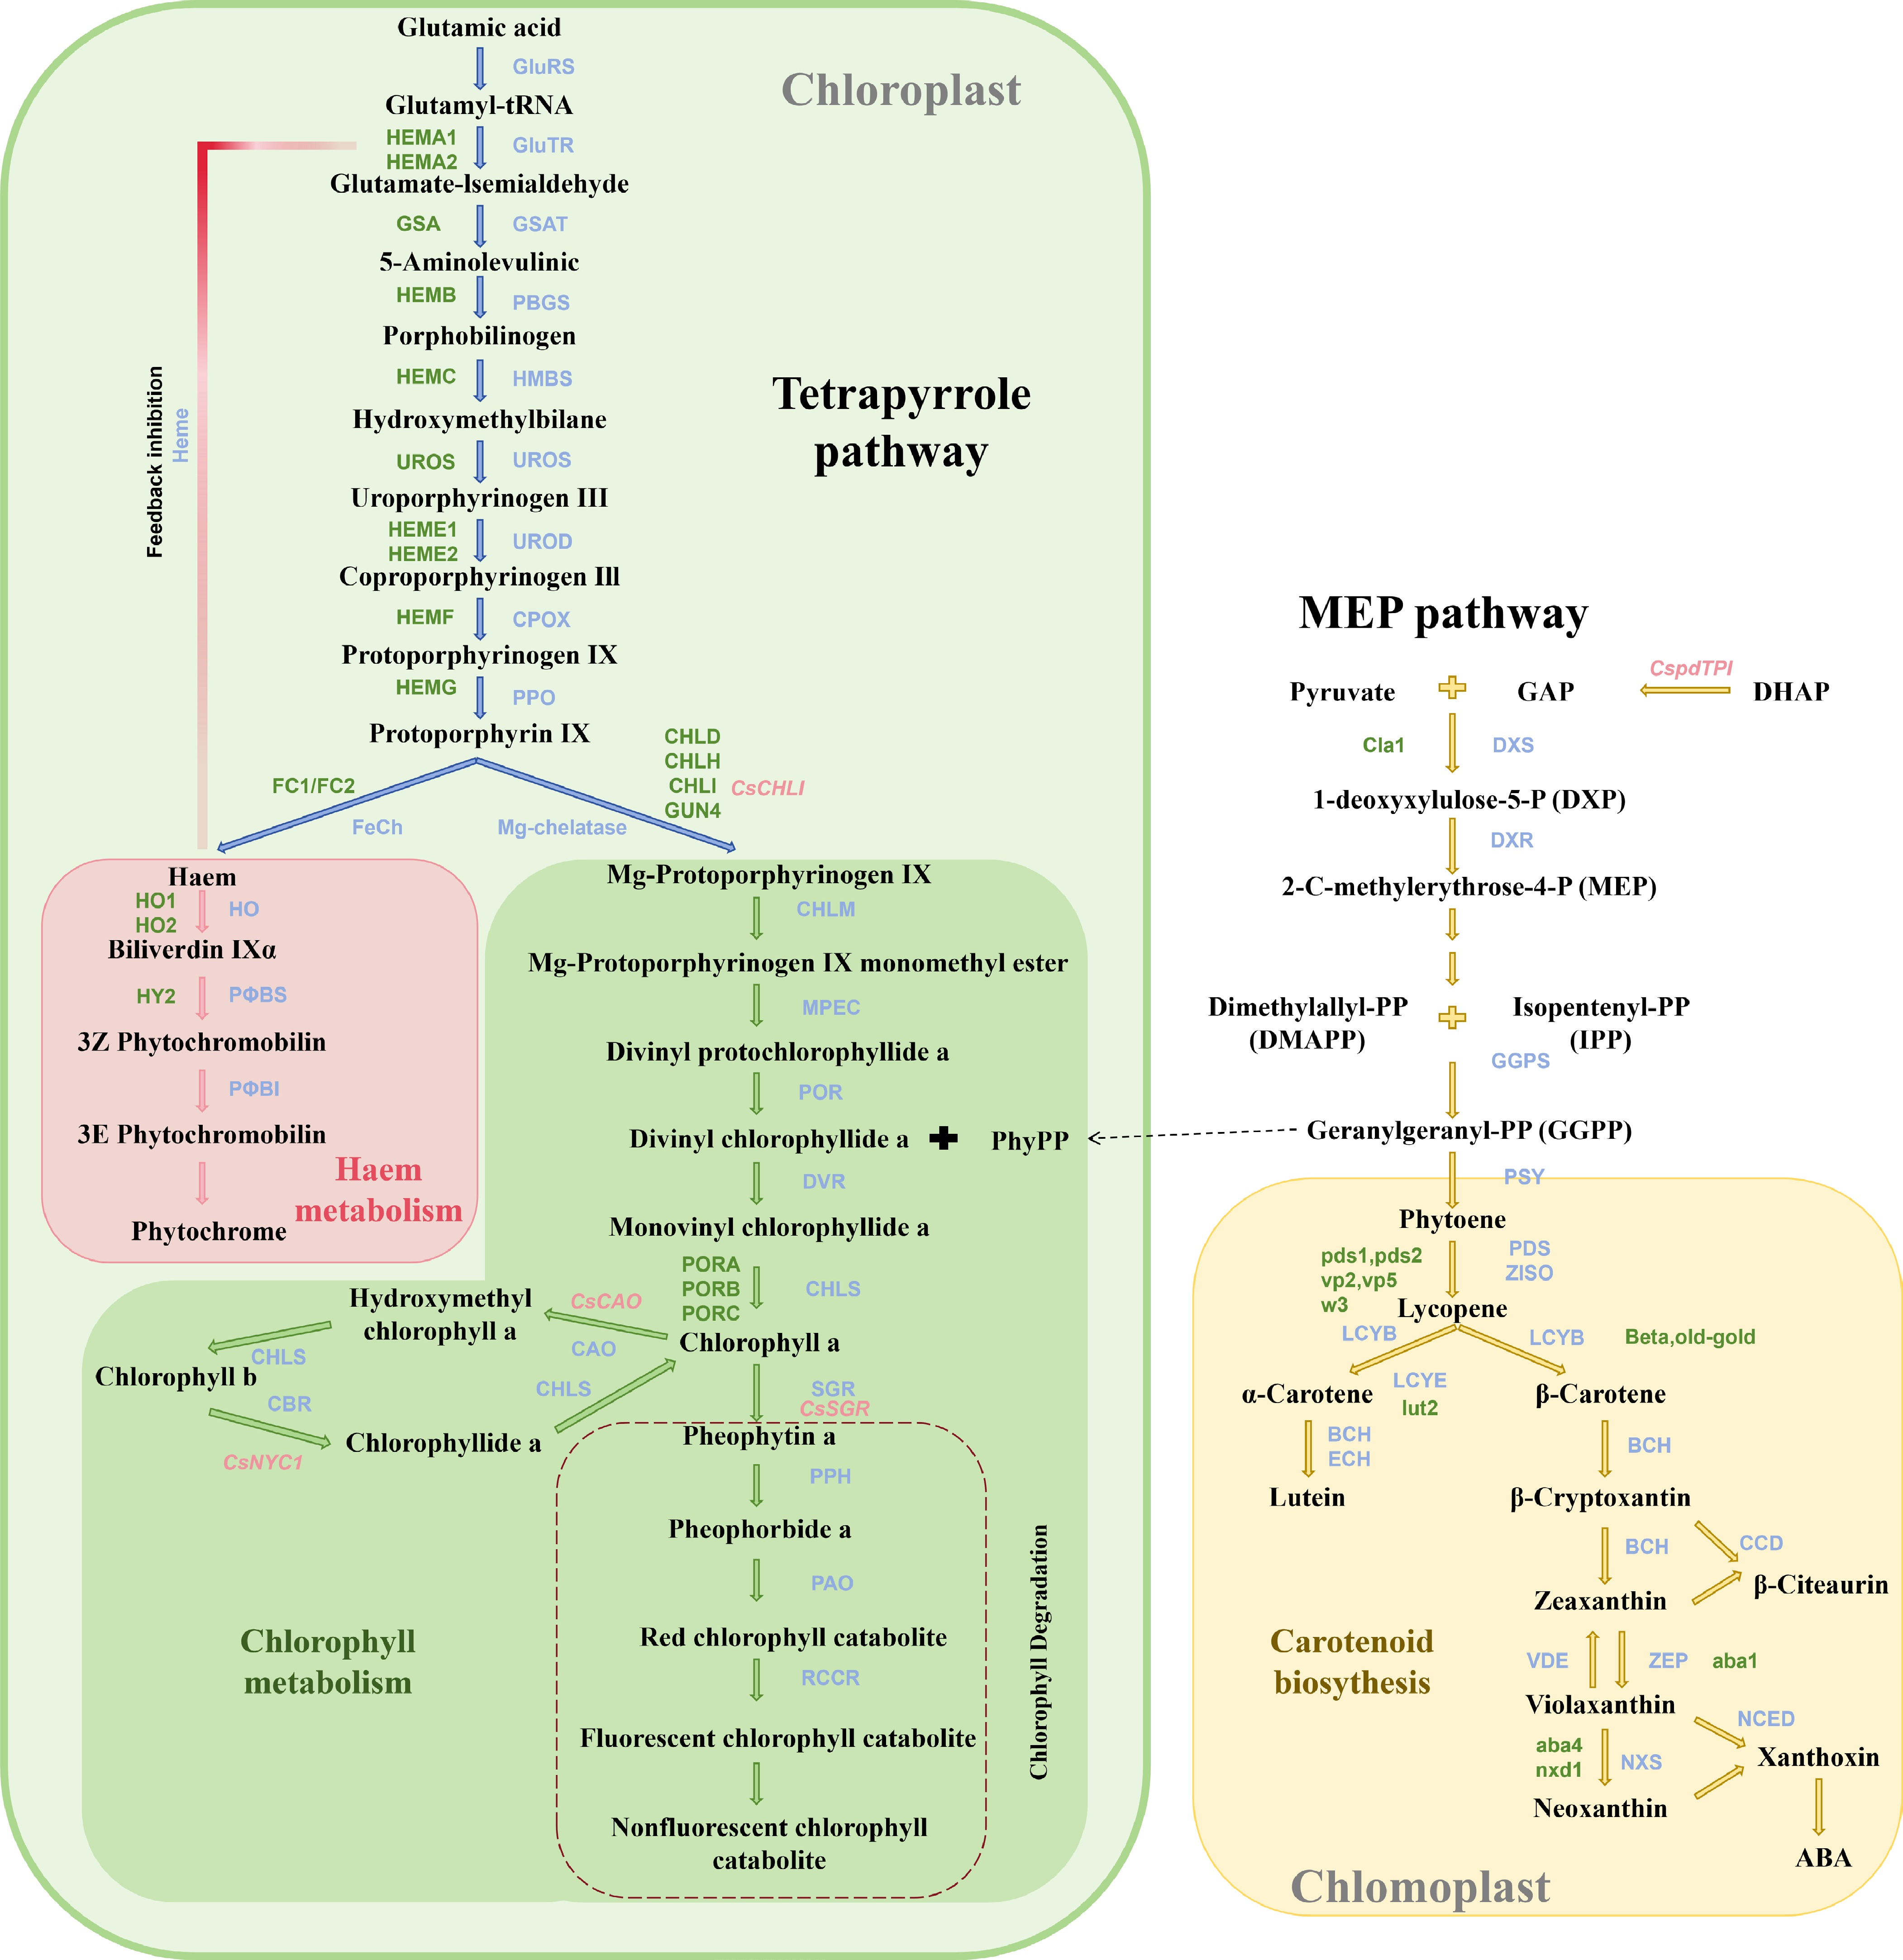
Figure 4.
The pigment metabolic network of chlorophyll, carotenoid, and heme pathways. The tetrapyrrole pathway begins with glutamic acid and branches at protoporphyrin IX to synthesize either haem (heme metabolism) or chlorophylls (chlorophyll metabolism). The chlorophyll metabolism module encompasses the synthesis of chlorophyll a and b, as well as their sequential degradation into nonfluorescent chlorophyll catabolites. Haem exerts a feedback inhibition on the early steps. The MEP and carotenoid biosynthesis pathways utilize pyruvate and GAP to produce various carotenes, xanthophylls, and abscisic acid (ABA). Genes were noted in green color, while enzymes were labeled in blue color. Genes highlighted in pink (e.g., CsCHLI, CsCAO, CspTPI) represent the key regulatory genes identified in cucumber (Cucumis sativus). Full names of enzyme abbreviations are listed below. GluRS: Glutamyl-tRNA synthetase acid; GluTR: Glutamyl-tRNA reductase; GSAT: Glutamate-1-semialdehyde aminotransferase; PBGS: Porphobilinogen synthase; HMBS: Hydroxymethyl-bilane synthase; UROS: Uroporphyrinogen III synthase; UROD: Uroporphyrinogen III decarboxylase; CPOX: Coproporphyrinogen III oxidase; PPO: Protoporphyrinogen IX Oxidase; FeCh: Ferrochelatase; HO: hemeo oxygenase; PΦBS: phytochromobilin synthase; PΦBI: phytochromobilin isomerase; Mg-chelatase: Protoporphyrin IX Mg-chelatase; CHLM: Mgprotoporphyrin IX methyltransferase; MPEC: Mg-protoporphyrin IX monomethylester oxidative cyclase; POR: protochlorophyllide oxidoreductase; DVR: Divinyl chlorophyllide a 8-vinyl reductase; CHLS: Chlorophyll synthase; CAO: Chlorophyllide a oxygenase; CBR: Chlorophyll b reductase; SGR: Mg-dechelatase; PPH: pheophytinase; RCCR: red chlorophyll catabolite reductase; DXS: 1-deoxy-D-xylulose-5-phosphate synthase; DXR: 1-deoxy-D-xylulose-5-phosphate reductoisomerase; GGPS: geranylgeranyl diphosphate synthase; PSY: Phytoene synthase; PDS: Phytoene desaturase; ZISO: ζ-carotene isomerase; LCYB: Lycopene-β-cyclase; LCYE: Lycopene-ε-cyclase; BCH: β-carotene hydroxylase; ECH: ε-carotene hydroxylase; CCD: Carotenoid cleavage dioxygenase; VDE: Violaxanthin de-epoxidase; ZEP: Zeaxanthin epoxidase; NXS: neoxanthin synthase; NCEDs: 9-cis-epoxycarotenoid dioxygenase.
The first reaction in chlorophyll synthesis takes place in the chloroplast stroma, where L-glutamyl-tRNA is catalyzed by glutamyl-tRNA synthetase to form 5-aminolevulinic acid (5-ALA). This is the rate-limiting step in chlorophyll biosynthesis. An early report on cucumber seedlings showed that two isoforms of GluTR (encoded by HEMA1 and HEMA2 genes) regulated green cucumber seedlings, with HEMA1 mRNA expression specialized for chlorophyll synthesis in photosynthetic tissues, while HEMA2 mRNA was dedicated to producing other porphyrins. This functional divergence indicates that plants can dynamically allocate metabolic flux within the tetrapyrrole pathway according to cellular requirements, leading to leaf color development. To ensure efficient chlorophyll biosynthesis, cpSRP43 directly stabilizes three key enzymes involved in the early and rate-limiting steps. Specifically, it binds to GluTR to facilitate 5-aminolevulinic acid (ALA) production and interacts with CHLH and GUN4 to regulate Mg2+ insertion via the magnesium chelatase complex[53]. In cucumber, CsSRP43 encodes a chlorophyll-signaling particle 43 kDa protein, which is a core component of the cpSRP complex, responsible for binding and protecting the chlorophyll synthesis limiting enzyme GluTR. Mutations in this gene cause chlorophyll synthesis to be blocked, GluTR to be unstable, chlorophyll precursors (PBG, Proto IX, etc.) content to be significantly reduced, and ALA to accumulate, suggesting that the conversion of ALA to bile pigment (PGB) is restricted[16].
In the second and third steps, 5-ALA is gradually converted into protoporphyrin IX (PPIX) by a series of enzymatic reactions in the chloroplast matrix, such as hydroxymethylbilane synthase, uroporphyrinogen III decarboxylase, and protoporphyrinogen IX oxidase. Following that, Mg2+ is inserted into PPIX, which is converted to magnesium protoporphyrin on the chloroplast membrane under the action of the magnesium chelate enzyme. Mg-chelatase consists of subunits of CHLI1, CHLI2, CHLD, CHLH, etc. Mutations affecting these subunits would result in chlorotic or yellow-green phenotypes due to impaired chlorophyll accumulation. In cucumber, a single nucleotide substitution occurred in the third exon of the CsCHLI, which led to a significant decrease in the activity of the magnesium chelate enzyme and could not efficiently catalyze the Mg2+ insertion reaction. As a result, the synthesis of chlorophyll a and chlorophyll b decreased significantly, the leaves appeared golden yellow, and they did not return to green[18]. Similar phenotypes have been widely reported in Arabidopsis thaliana, rice, and Chinese cabbage, underscoring the conserved role of this enzyme in chlorophyll biosynthesis[54−56].
Lastly, chlorophyllide was converted into chlorophyll a and chlorophyll b, which can be transformed into each other through redox reactions to form a chlorophyll cycle on the thylakoid membrane. Protochlorophyllide-dependent processes are essential for chlorophyll a/b formation. The protochlorophyllide-dependent translocon component 52 gene (CsPTC52, often associated with POR complexes) was proposed to be the causal gene underlying cucumber yellow green leaf 3 (ygl3) mutants. It could facilitate the conversion of protochlorophyllide to chlorophyllide under light conditions. Disruption of this process leads to the accumulation of phototoxic intermediates and severe albino phenotypes, reflecting the sensitivity of tetrapyrrole metabolism to enzymatic imbalance. A recent study on Peony PlPTC52 showed that it was responsible for high-temperature-mediated chlorophyll loss[57]. However, the function of CsPTC52 required further validation in cucumber. Moreover, chlorophyllide a oxygenase (CAO) catalyzes the conversion of chlorophyll a to chlorophyll b, thereby regulating the composition of light-harvesting complexes. The CsCAO was proposed to be the causal gene underlying the yellow leaf 2 (yl-2) mutant identified from EMS mutagenesis[19]. Mutations in CAO homologs have been reported in a number of plants, such as AtCAO in Arabidopsis thaliana, OsCAO1 in rice, and CmCAO in melon (Cucumis melo L.), respectively[58−60].
In addition to chlorophyll biosynthesis, the tetrapyrrole pathway also gives rise to heme, an essential cofactor involved in electron transport, redox regulation, and retrograde signaling. The metabolic flux between the chlorophyll and heme branches is tightly controlled at the protoporphyrin IX node, primarily through the competing activities of Mg-chelatase and Fe-chelatase. In several plant species, mutations affecting heme biosynthesis have been shown to cause leaf color abnormalities[61]. For example, defects in ferrochelatase or other heme-associated enzymes in Arabidopsis thaliana, rice, and tomato result in chlorotic or pale-green phenotypes, like mutant HY1 (Arabidopsis thaliana), ygl2 (Oryza sativa L.), and yg-2 (Solanum lycopersicum)[62−64]. Through the investigation of the Brassica napus chlorophyll-deficient mutant ygl, BnaC07.HO1 was identified as a critical regulator of chlorophyll metabolism. BnaC07.HO1, which encodes a heme oxygenase, participates in heme catabolism and dynamically regulates the chlorophyll biosynthesis rate through a feedback inhibition pathway to ensure photosynthetic homeostasis[65]. So far, leaf color mutants directly linked to heme biosynthesis have not yet been reported in cucumber. This absence may reflect limited genetic resolution or functional redundancy within the pathway. Future studies integrating high-resolution mapping and metabolite profiling may uncover hidden variation in heme-related genes and clarify their contribution to leaf color regulation in cucumber.
Chlorophyll degradation is equally important as chlorophyll synthesis for leaf color maintenance. It starts with the removal of magnesium ions by chlorophyll a under the catalysis of magnesium-dechelatase to form Pheophytin A. Under the action of the enzyme pheophorbide a oxygenase (PAO), the porphyrin ring structure is opened to form a linear pheophytin a, which is further converted into red chlorophyll degradation products. The red product is catalyzed by red chlorophyll degradation product reductase to produce a primary fluorescent chlorophyll degradation product, and finally undergoes a non-enzymatic transformation, becoming a stable, colorless, nonfluorescent chlorophyll degradation product (Fig. 4). STAYGREEN (SGR) encodes magnesium dechelatase, a key regulator of chlorophyll breakdown, while NON-YELLOW COLORING 1 (NYC1) encodes Chl b reductase that participates in the conversion of Chl b to 7-hydroxymethyl Chl, and it has been demonstrated to interact with SGR[66]. Under leaf senescence or adversity stress, cucumber CsSGR protein is induced to express and interact with the light-harvesting complex of CsNYC1 and photosystem II to jointly form a protein complex that catalyzes chlorophyll decomposition, resulting in chlorosis and yellowing of leaves. After its function is inhibited or destroyed, the chlorophyll degradation pathway is blocked, and the leaves remain green under stress, showing a Staygreen phenotype[67,68]. In other crops such as rice, the leaf color mutants reported to be associated with chlorophyll degradation are usually evergreen or stay green[69]. Furthermore, such a Staygreen phenotype was also reported to compromise disease resistance in cucumber and soybean[67,70].
Carotenoid metabolism and metabolic support
-
Carotenoids serve dual roles as accessory pigments in light harvesting and as essential photoprotective molecules that quench excess energy and ROS[71]. Leaf color phenotypes can arise from shifts in relative pigment ratios: when the relative content of chlorophyll is low, plant leaves will show carotenoid color. Plant carotenoid biosynthesis initiates via the plastidial methylerythritol phosphate (MEP) pathway, generating the C5 precursor isopentenyl pyrophosphate (IPP), which is assembled into the C20 intermediate geranylgeranyl pyrophosphate (GGPP). In the first dedicated and rate-limiting step, phytoene synthase (PSY) condenses two GGPP molecules into 15-cis-phytoene. This colorless intermediate undergoes sequential dehydrogenation and isomerization--catalyzed by PDS, ZDS, Z-ISO, and CRTISO—to yield all-trans lycopene. At this critical branch point, lycopene is cyclized by LYCB and LCYE into α- and β-carotene, which are subsequently hydroxylated and epoxidized by enzymes like BCH and CYP97 to form xanthophylls (e.g., lutein, zeaxanthin, and violaxanthin). Although genes directly involved in carotenoid biosynthesis have not been functionally characterized in cucumber leaf color mutants, a few disruptions in carotenoid-associated processes related to carotenoid turnover have affected leaf coloration.
In the ygl1 mutant, missense mutations in four tandemly duplicated 13-lipoxygenase (LOX) genes lead to impaired enzyme function[15]. LOXs are involved in lipid oxidation and play important roles in oxylipin metabolism and membrane remodeling. Disruption of CsLOX activity is associated with reduced carotenoid degradation, resulting in carotenoid accumulation and a concomitant decrease in chlorophyll content[15]. This imbalance enhances the visual prominence of yellow pigments, leading to a chlorotic phenotype[15]. Similarly, the critical role of carotenoid metabolism in determining leaf color has been widely documented in other crops, such as the pepper leaf yellowing mutant yl1[72].
The plastid isoform of triose phosphate isomerase (pdTPI), a key enzyme in the Calvin cycle, catalyzes the reversible interconversion between dihydroxyacetone phosphate (DHAP) and glyceraldehyde-3-phosphate (GAP). GAP is a crucial starting material in the MEP pathway. By regulating the balance of triose phosphates, TPI influences the supply of precursors for the MEP pathway, which generates isoprenoid intermediates required for carotenoid synthesis. A yellow-leaf mutant yl2.1 with no green-revertant phenotype was reported for the causal gene, which encodes pdTPI[73]. The mutation of CspdTPI leads to inactivation of pdTPI, and insufficient GAP production causes leaf yellowing. Mutations in plastid TPI can therefore lead to reduced carotenoid levels, impaired photoprotection, and secondary chlorophyll loss.
Similarly, enzymes involved in cofactor biosynthesis, such as 5-amino-6-(5-phosphoribosylamino) uracil reductase (a key enzyme in riboflavin biosynthesis), may indirectly affect carotenoid metabolism by modulating redox cofactors (e.g., FAD, FMN) required for enzymatic reactions. This illustrates how disruptions in seemingly peripheral metabolic pathways can propagate into pigment biosynthesis networks.
Transport processes and integrated networks in pigment regulation
-
In cucumber, some leaf color mutant genes do not specifically participate in a particular step of chlorophyll and carotenoid metabolism, but they operate in the regulatory network, such as v-2 and yc412[6,74]. The causal gene for mutant v-2, which showed virescent phenotypes, encodes transport inhibitor response 1-like protein, which is an F-box protein. F-box protein is a key component in the growth signaling pathway and is involved in regulating ubiquitination and degradation of Aux/IAA proteins. After a gene mutation, the function of the F-box protein is impaired, preventing normal degradation of Aux/IAA proteins, resulting in persistent suppression of the ARF transcription factor, thereby preventing the initiation of transcription of chlorophyll synthesis-related genes[6].
Another spontaneous mutant, yc412, exhibited yellow cotyledons and a lethal phenotype, leading to plant death about 10 d after germination. The causal gene Csyc encodes a yellow stripe-like (YSL) transporter, which is mainly responsible for the transport of iron ions (Fe3+). Iron is a necessary cofactor for several key enzymes in chlorophyll synthesis, and iron deficiency affects the activity of chlorophyll synthesis-related enzymes[74].
Nuclear–cytoplasmic communication
-
Chloroplast biogenesis and function depend on tight coordination between the nuclear and plastid genomes. Although chloroplasts contain their own genetic system, encoding a small subset of proteins, the vast majority of chloroplast proteins are nuclear-encoded, synthesized in the cytosol, and subsequently imported into the organelle. It is estimated that chloroplasts harbor more than 3,000 proteins, yet only ~5% are plastid-encoded, whereas over 90% are encoded by nuclear genes. This asymmetry necessitates extensive nuclear-cytoplasmic communication, including both anterograde (nucleus-to-plastid) and retrograde (plastid-to-nucleus) signaling pathways, to ensure coordinated gene expression and proper chloroplast development[75,76] (Fig. 5).
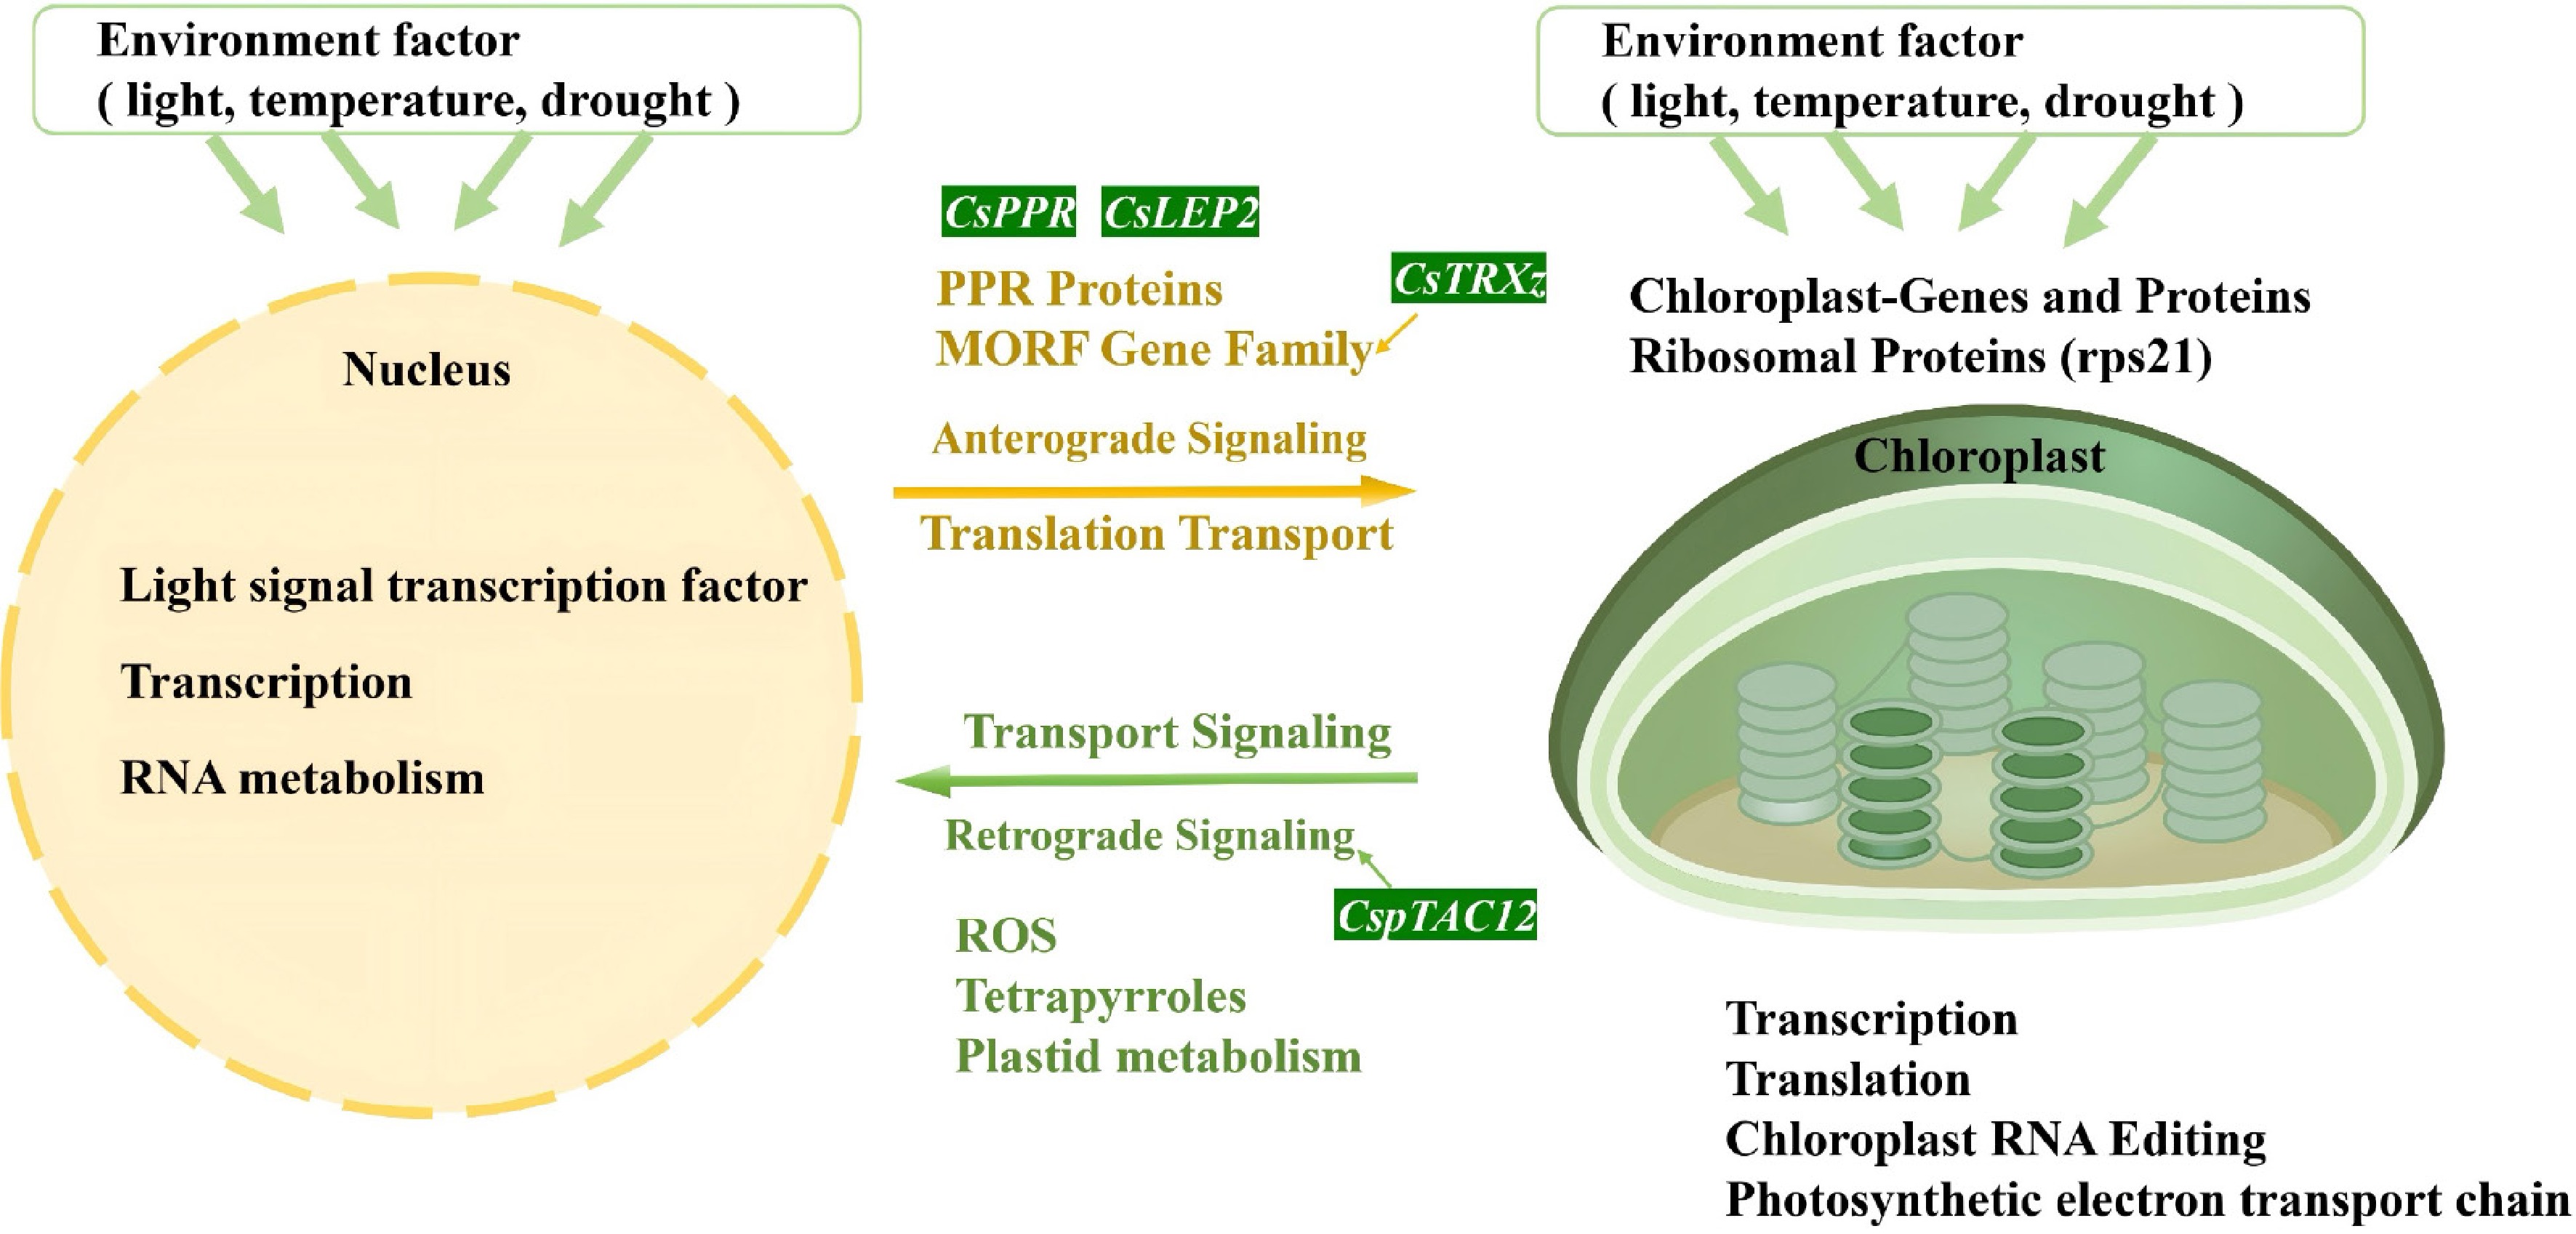
Figure 5.
Schematic model of nuclear-cytoplasmic communication. An environmental stimulus (e.g., light, temperature) is perceived by the nucleus and communicated to the chloroplast via anterograde signaling. During this process, specific nuclear-encoded regulators, such as PPR proteins (e.g., CsPPR), MORF (plastid multiple organellar RNA editing factors) family members, and ribosomal proteins (e.g., rps21), are transported into the plastid to govern chloroplast RNA editing and translation. In contrast, metabolic shifts (e.g., ROS, tetrapyrroles) or translation defects generated by the chloroplast produce retrograde signals. These signals are transduced back to the nucleus, causing changes in nuclear gene expression. Genes highlighted in a green background (e.g., CsPPR, CsLEP2) represent the key regulatory genes identified in cucumber (Cucumis sativus).
In cucumber, although studies on nuclear-cytoplasmic communication that regulate leaf color remain limited, emerging evidence highlights the importance of nuclear-encoded factors controlling plastid gene expression at multiple levels, leading to leaf color mutants. A representative example is the yl-5 mutant, in which leaf pale yellowing is caused by a mutation in CsaV3_3G027140, identified through Tnt-1 insertion[20]. This gene encodes the plastid 30S ribosomal protein S21 (rps21), a homolog of the Arabidopsis thaliana LOW PHOTOSYNTHETIC EFFICIENCY2 (LPE2) gene[77]. rps21 is a structural component of the 30S ribosomal subunit that is part of the 70S-type chloroplast ribosome[78]. Disruption of rps21 impairs the function of the 70S ribosome in chloroplasts, leading to defective translation of photosynthesis-related proteins[79]. Importantly, studies in Arabidopsis further demonstrate that LPE2/rps21 deficiency not only affects plastid translation but also triggers broader nuclear responses[77]. Loss of LPE2 leads to reduced accumulation of photosynthetic proteins and alters the expression of nuclear genes associated with photosynthesis and metabolism[77]. These findings suggest that plastid translational defects can act as signals to reprogram nuclear gene expression, linking chloroplast functional status with cellular metabolic regulation.
The cucumber pentatricopeptide repeat protein CsPPR, which functions in plastid RNA editing, was identified, leading to leaf color asymmetry in reciprocal hybrids between Cucumis sativus and C. hystrix dysfunction of CsPPR may be associated with impaired post-transcriptional regulation of plastid transcripts, providing new insights into the regulatory mechanisms of asymmetric phenotypes in plant reciprocal crosses[80]. Both cases of rps21 and CsPPR are related to anterograde signaling, but retrograde signaling in regulating leaf color mutants has not been reported in cucumber.
Other examples identified in other crops also demonstrated the critical role of nuclear-cytoplasmic communication in coordinating chloroplast development, resulting in leaf color differential. For instance, the mutation of gene members in the multiple organellar RNA editing factor (MORF), such as atmorf2, atmorf9, osmorf9-1, osmorf9-1, and AgWp1, leads to albino seedlings and white-spot leaf phenotypes in Arabidopsis, rice, and celery (Apium graveolens)[81−83]. The loss of MORF genes was proposed to impair the biogenesis of plastidic ribosomes and the editing and splicing of specific plastidic RNA molecules. In rice, OsMORF9 was identified interacting with the DUA1 gene, which is a member of the pentatricopeptide repeat (PPR) family of proteins[83]. DUA1 specifically mediates the editing of plastid-encoded transcripts such as rps8 under low-temperature conditions, and its disruption leads to defective chloroplast development, resulting in weak and yellowing seedlings[84]. The activity and stability of DUA1 are further modulated by its interacting partner WSP1, highlighting the importance of multi-protein complexes in plastid RNA metabolism. Importantly, natural variation in DUA1 is associated with differences in chlorophyll accumulation and chilling tolerance among rice cultivars, indicating that nuclear–cytoplasmic communication via plastid RNA editing is tightly linked to environmental adaptation.
Together, these findings reinforce that post-transcriptional regulation of plastid gene expression, particularly RNA editing mediated by nuclear-encoded factors, represents a conserved and dynamic mechanism underlying chloroplast development and its coordination with nuclear gene expression across plant species.
-
Recent studies have substantially advanced understanding of the genetic basis of leaf color variation in cucumber, with 24 leaf color loci now mapped across six chromosomes and a growing number of causal genes functionally characterized. These genes primarily modulate leaf color through chlorophyll biosynthesis and chloroplast development pathways, involving rate-limiting enzymes such as CsCHLI and CsSRP43[16,18]. Furthermore, components of the chloroplast inner membrane translocon (e.g., CsTIC21), protein folding quality control systems (e.g., CsVYL, CsFtsH), and plastid-encoded RNA polymerase (PEP) complex-related factors (e.g., CsSIG2, CsTRXZ) have been shown to play decisive roles in maintaining chloroplast structural integrity during early development[3,5,9,12,14]. Within the pigment metabolic network, progress includes the identification of genes governing chlorophyll degradation (e.g., CsSGR, CsNYC1) and carotenoid-related turnover (e.g., CsLOX), clarifying how shifts in pigment composition give rise to distinct leaf color phenotypes[15,66]. In parallel, emerging work on nuclear-cytoplasmic communication, including the identification of CsPPR and rps21/yl-5, has begun to reveal how nuclear-encoded factors coordinate plastid gene expression to shape leaf coloration[20,80]. Together, these advances provide an increasingly detailed genetic framework spanning chloroplast development, pigment metabolism, and nuclear-plastid signaling, and lay essential groundwork for the breeding applications discussed below.
The distinctive phenotypic spectrum of cucumber mutants
-
Despite significant progress in identifying and characterizing leaf color-related genes in cucumber, several key challenges and knowledge gaps remain. First, current studies are heavily biased toward genes with strong and visually distinct phenotypes, such as albino and virescent mutants[3,4,12]. In contrast, genes with subtle regulatory roles, particularly those involved in fine-tuning pigment homeostasis or environmental responsiveness, are likely underrepresented. This bias limits our understanding of the quantitative and dynamic nature of leaf coloration, and contributes to the markedly uneven phenotypic spectrum of cucumber mutants relative to other crops, discussed further below. Future efforts should prioritize the identification of quantitative trait loci (QTL) and minor-effect genes using high-resolution mapping populations and genome-wide association studies.
Phenotypically, cucumber mutants exhibit a distinct distribution compared to other crops. Since the 1980s, rice leaf color mutations have been categorized into eight types, including albino, greenish-white, white emerald, and light green[85], and thermos-sensitive phenotypes have been extensively characterized within this spectrum, providing detailed insights into temperature-dependent chloroplast regulation[86]. In cucumber, by contrast, mutants are unevenly distributed: virescent and greenish phenotypes are common, whereas variegated and temperature-sensitive mutants are rare with only one variegated case (csvl)[10] and two temperature-sensitive cases (PSM004_DVL, hs1)[9,11].
Several non-exclusive explanations may account for this pattern. First, many cucumber virescent genes (e.g., CsVYL, CsSIG2, CsTRXz, CsCNGCs) act on broadly conserved, rate-limiting steps of chloroplast protein import, PEP-dependent transcription, or Ca2+ signaling rather than causing complete pathway blockade. Because these processes are most limiting in young, rapidly dividing tissue with high demand for chloroplast biogenesis, partial loss-of-function alleles tend to produce a transient developmental delay that is compensated as the leaf matures and metabolic redundancy increases, generating the characteristic 'yellow-then-green' trajectory shared by v-1, v-2, CsVYL, and Csvl-6 mutants[3−6]. Second, ascertainment bias likely contributes: virescent and yellow-green phenotypes are non-lethal, fertile, and easily scored at the seedling stage, making them disproportionately easy to recover and propagate in mutagenesis populations, whereas more severe phenotypes such as albino mutants often require specialized propagation methods such as grafting[50]. Third, variegation in other species frequently arises from stochastic, cell-autonomous defects—such as mosaic plastid genome instability, heteroplasmy, or transposon-mediated silencing—that segregate independently of simple Mendelian nuclear mutations; such mechanisms may be comparatively rare among the genetic backgrounds sampled by standard cucumber mutagenesis programs, which could explain why only a single variegated phenotype has been reported to date. Finally, the apparent rarity of temperature-sensitive mutants in cucumber, relative to the extensively characterized thermo-sensitive spectrum in rice[86], may partly reflect limited screening under variable thermal conditions rather than a true absence of underlying genetic variation. Disentangling these biological and methodological explanations offers an interesting entry point for understanding both the genetic architecture and breeding history of leaf color variation in cucumber.
Gaps in functional validation and whole-plant characterization
-
Although many candidate genes have been identified, functional validation remains insufficient. A substantial proportion of reported genes are supported only by mapping, expression profiling, or homology-based inference. Direct genetic evidence is limited, such as complementation tests, CRISPR/Cas-mediated validation, or allelic analysis. As a result, the extent to which these genes show divergent gene function compared with model plants Arabidopsis or other crops remains unclear. Establishing robust and standardized functional validation pipelines will be critical for strengthening causal inference in cucumber and enabling cross-species comparisons.
Current research largely adopts a gene-by-gene perspective and lacks a whole-plant framework. Most studies focus on seedling-stage phenotypes, particularly early leaf coloration, while overlooking gene functions during later developmental stages. This limitation is especially relevant given that many virescent mutants gradually recover greening, suggesting dynamic and stage-dependent regulatory mechanisms (e.g., v-1; PSM004_DVL)[4,9]. Conversely, non-recovering mutants often exhibit persistent defects that may affect overall plant growth and reproductive development, including fruit traits (e.g., gl; ygl3)[18,87]. However, these broader physiological consequences remain poorly explored, underscoring the need to evaluate gene function not only across developmental stages but also across organs.
While chloroplast development and pigment metabolism networks are typically shared across plant organs, the limited data available in cucumber suggest that this sharing does not always translate into consistent pigmentation outcomes. Of the 24 reported leaf color mutants, five mutants died at the seedling stage and never reached fruiting. Among the remainder, only five studies explicitly reported that fruit color matched the corresponding leaf phenotype (e.g., gl; v-2; yf; se59; ygl3)[6,8,16,18,87]. For the rest, fruit pigmentation was either not assessed or not reported, making the tree prevalence of organ-specific divergence difficult to estimate. Increasing evidence points to spatial specificity in pigment regulation. For instance, the cucumber CsAPRR2 gene regulates fruit chlorophyll accumulation, resulting in white fruit phenotypes without affecting leaf coloration[88]. Similarly, genes involved in carotenoid metabolism (e.g., CsOre) predominantly influence fruit flesh color rather than leaf pigmentation[89]. By contrast, pleiotropic effects on stem or flower pigmentation have not yet been systematically examined for any cucumber leaf color gene, representing a further blind spot in the current literature. Together, these observations highlight the importance of tissue-specific expression and regulatory divergence, suggesting that pigment biosynthesis and chloroplast development are differentially controlled across organs. Dissecting the molecular basis of such spatial regulation will be critical for linking leaf- and fruit-related traits within a unified framework.
Emerging frontiers, alternative pigments, physiology, and regulatory integration
-
Beyond chlorophyll and carotenoids, anthocyanins (flavonoid-derived secondary metabolites) are also well known to influence leaf color in ornamental plants and model species like Arabidopsis (e.g., the MYB transcription factor PAP1 mediates purple pigmentation)[90]. In cucumber, however, no leaf-color mutant has yet been attributed to anthocyanin biosynthesis; the only reported role of anthocyanins is in determining fruit black spine[91]. Given that anthocyanin pathway defects often result in distinct leaf phenotypes in other crops, whether comparable mechanisms might underlie as-yet-undiscovered leaf color variation in cucumber remains an open question.
The physiological and agronomic consequences of leaf color variation also warrant greater attention. Leaf coloration usually determines the photosynthetic capacity of source organs, which in turn affects the distribution of assimilates and fruit development. Severe etiolated or albino mutations often reduce total photosynthetic productivity, resulting in slow growth and development, delayed flowering, and reduced yield[92]. Particularly, Zhou et al. provided an approach that uses grafting to rescue the albino phenotypes, indicating that systemic physiological support from photosynthetically competent rootstock can compensate for chloroplast defects in the scion[50]. This finding highlights the importance of whole-plant integration and suggests that some consequences of chloroplast dysfunction are not strictly cell-autonomous.
The integration of different regulatory layers, including chloroplast development, pigment metabolism, and nuclear-cytoplasmic communication, remains insufficient. Most studies focus on individual pathways, whereas leaf color phenotypes often arise from complex interactions among metabolic, genetic, and environmental factors. In particular, nuclear-cytoplasmic communication represents a largely unexplored frontier in cucumber. While studies in model plants have revealed the importance of retrograde signaling in coordinating chloroplast and nuclear gene expression[93], similar mechanisms have not been systematically investigated in cucumber. Elucidating these pathways will provide critical insights into how chloroplast dysfunction influences whole-cell physiology. Systems-level approaches, such as multi-omics integration (transcriptomics, proteomics, metabolomics), will be essential to construct comprehensive regulatory networks[94].
Application in breeding and fundamental research
-
The application of leaf color mutations in breeding remains underutilized. Due to their high visibility and early manifestation, leaf color traits serve as convenient morphological markers for seedling-stage selection, facilitating rapid identification of off-type individuals and improving the efficiency of hybrid seed production[95]. More recently, causal genes underlying leaf color mutations have been further exploited as phenotypic markers in haploid induction systems in maize, foxtail millet (Setaria italica), and other crops[96,97]. By linking visible leaf color phenotypes with haploid-specific genetic backgrounds, these systems enable efficient identification and screening of haploid individuals at early developmental stages[96]. This approach greatly reduces the reliance on labor-intensive cytological or molecular assays, thereby accelerating doubled haploid breeding pipelines and improving selection efficiency. The sources of leaf color-related genes summarized in this review could be the gene pool adopted for cucumber haploid induction[98].
Beyond their practical utility in breeding, leaf color mutants also represent powerful experimental materials for fundamental research. Because leaf coloration is tightly linked to photosynthesis and chloroplast function, these mutants provide direct entry points for dissecting plant physiological and molecular processes[61]. For instance, characterizing the reversible yellowing tomato mutant gret1 revealed that the DYW-type protein SlPPR138 governs rpoC1 RNA editing, highlighting a critical post-transcriptional mechanism that controls PEP assembly and photosynthetic gene expression during chloroplast development[99].
Taken together, leaf color mutations represent a unique intersection between practical breeding tools and mechanistic research resources, highlighting their importance for advancing cucumber improvement and plant biology research more broadly. Future research would benefit from moving beyond gene identification toward integrative and application-oriented studies, bridging the gap between molecular mechanisms and breeding practice. Such efforts will not only deepen our understanding of chloroplast biology but also contribute to the sustainable improvement of cucumber and other horticultural crops.
We thank the high-performance computing platforms at the Bioinformatics Center of Nanjing Agricultural University for supporting this project. This study was supported by the Fundamental Research Funds for the Central Universities (Grant Nos KJYQ2024026, KJYQ2025022, KJYQ2026017); the Fund for Seed Industry Revitalization Project (Grant No. JBGS[2021]070); Open Fund of the Key Laboratory for Quality Regulation of Tropical Horticultural Crops of Hainan Province (Grant No. HNZDSYS(2025)-12) and a project funded by the Priority Academic Program Development of Jiangsu Higher Education Institutions.
-
The authors confirm contribution to the paper as follows: study conception and design: Wang Y, Lou Q; literature review: Shu J, Wang Y; figure preparation: Shu J; draft manuscript preparation: Shu J, Wang Y. All authors reviewed the results and approved the final version of the manuscript.
-
All data generated or analyzed during this study are included in this published review and its supplementary information files.
-
The authors declare that they have no conflict of interest.
-
accompanies this paper online at: https://doi.org/10.48130/vegres-0026-0022.
- Supplementary Table S1 Summary information of all reported mutants for cucumber leaf color variation (updated to May 2026).
- Copyright: © 2026 by the author(s). Published by Maximum Academic Press, Fayetteville, GA. This article is an open access article distributed under Creative Commons Attribution License (CC BY 4.0), visit https://creativecommons.org/licenses/by/4.0/.
-
About this article
Cite this article
Shu J, Lou Q, Wang Y. 2026. Molecular mechanisms of leaf color variation in cucumber (Cucumis sativus): from chloroplast biogenesis to metabolic and signaling networks. Vegetable Research 6: e029 doi: 10.48130/vegres-0026-0022 

Molecular mechanisms of leaf color variation in cucumber (Cucumis sativus): from chloroplast biogenesis to metabolic and signaling networks
- Received: 09 May 2026
- Revised: 21 June 2026
- Accepted: 08 July 2026
- Published online: 24 August 2026
Abstract: Leaf color mutants are invaluable genetic resources for deciphering the mechanisms of pigment metabolism, chloroplast biogenesis, and photosynthesis, while also offering a reference for cucumber breeding. However, the regulation of leaf coloration in cucumber is a highly complex trait driven by diverse regulatory networks, involving chloroplast structural integrity, pigment biosynthesis pathways (chlorophyll, carotenoids, and heme), and intricate nuclear-cytoplasmic signaling. Recently, substantial breakthroughs have been achieved in elucidating the genetic and molecular basis of leaf color variation in this vital crop. Here, we systematically synthesize recent advances in the identification, mapping, and functional characterization of leaf-color-related genes in cucumber. We highlight key genetic determinants governing pigment metabolism and chloroplast development, critically discuss their regulatory networks and pleiotropic effects on plant growth, and provide perspectives on future research directions to accelerate molecular breeding in cucumber.
-
Key words:
- Cucumber /
- Leaf color mutant /
- Molecular mechanism /
- Chloroplast biogenesis /
- Chlorophyll metabolism