




-
Microbial electrobiotechnology has emerged as a powerful interdisciplinary field at the intersection of microbiology, electrochemistry, and process engineering. It has the potential to address current industrial and social challenges in relation to the United Nations Sustainable Development Goals[1]. It exploits the ability of electroactive microorganisms to exchange electrons with solid electrodes, enabling the direct coupling of microbial metabolism to electrical circuits. This unique capability opens up new possibilities for the sustainable production of chemicals, the generation of bioenergy, the capture of carbon dioxide, the treatment of wastewater, and the recovery of resources[2]. Technologies such as microbial fuel cells and microbial electrosynthesis systems show how bio-electrochemical platforms can convert waste streams or carbon dioxide into electricity or valuable products. Microbial electrobiotechnology supports the concept of a circular bioeconomy and climate-neutral production strategies.
Despite its significant potential, transitioning microbial electrobiotechnology into real applications remains a major challenge. A key factor contributing to this bottleneck is the absence of scalable reactor systems capable of reliably integrating and controlling both electrochemical and biotechnological parameters across different scales[3]. Unlike conventional bioreactors, bio-electrochemical reactors must satisfy the requirements of microbial cultivation, such as mono-septic conditions, suitable mass transfer, pH, temperature control, and nutrient supply, as well as the constraints of electrochemical systems. These include uniform current distribution, controlled electrode potentials, low ohmic resistance, efficient utilization of the electrode surface, and minimized energy losses. Achieving this dual optimization becomes increasingly complex during scaling up, where gradients in substrate concentration, redox potential, and current density can severely affect microbial activity and process performance.
Therefore, developing standardized, scalable reactor options is essential for advancing the field. Various authors have already modified the laboratory-scale bioreactor to bridge the gap between the requirements of microbial cultivation and electrochemistry[4−7]. In addition to large-scale reactors, milliliter-scale systems are essential because they facilitate rapid parameter optimization and statistically robust experimentation while significantly reducing material consumption and operational costs. Such screenings are typically carried out in H-cells. Although H-cells are widely used in laboratories due to their simple design, low cost, and ease of implementation, they were originally developed for fundamental electrochemical studies rather than for optimizing bioprocesses. Consequently, they have several limitations, including high internal resistance, poorly defined hydrodynamics, limited scalability, and non-representative mass transfer conditions[8]. These limitations restrict the transferability of results to technically relevant reactor systems. Replacing classical H-cells with milliliter-scale electro-bioreactors improves control over mass transfer, electrode geometry, and current distribution. This generates scalable, quantitatively transferable data rather than purely exploratory results. The aim of this study is therefore to electrify a small-scale commercial bioreactor system as an alternative to H-cells.
For electrification, an affordable small-scale system was chosen, which was constructed not just for scientists but also for school kids or hobbyists: the Pioreactor®[9]. The main parts of this reactor system are 3D-printable, and the software runs on a Raspberry Pi computer. Overall, all the parts are kept low-cost and affordable for a reactor with various configuration options; for example, anaerobic or continuous fermentation modes adjusted with two peristaltic pumps[10−12]. It's an easily built and easy-to-run reactor for simple tasks like growing baker's yeast in an apple juice suspension or, on the other hand, growing lab strains in turbidostatic mode for long periods of time to adapt them to different process conditions. With built-in photodiodes for optical density measurement, a magnetic stirrer, a heating pad, liquid handling, and an intuitive online platform for monitoring and control of the reactor, as well as the possibility to creating a cluster of several reactors running in parallel, the reaction system can be regarded as an ideal platform reactor for further development in the field of electrobiotechnology (Pioreactor, Waterloo, Canada). A fitting model organism ideally covers different configurations and different electrobiotechnological systems it can be used in. As electrobiological applications have also reached bacteria which are not classically viewed as electroactive, Cupriavidus necator has also been applied in electro-autotrophic approaches. Even though C. necator does not interact directly with an electrode, anodic respiration has just recently been discovered, as C. necator is able to use mediated electron transfer (MET)[13,14]. With a wide substrate spectrum containing heterotrophic as well as autotrophic carbon and energy sources, these bioelectrical applications can be realized. As a first example, the electro-autotrophic cultivation with C. necator by the utilization of flue gas was shown[15]. A second application, using fructose as a heterotrophic carbon source with the anode serving as an electron acceptor, was introduced by Gemünde et al.[13]. With this fitting model organism and an ideal small-scale reactor system to be electrified, there might be a possible alternative for H-cells.
Next to the need for a small-scale bioelectrical system (BES), another need occurred in electrobiotechnology. It's not always process or reactor limitations that keep the total efficiency low, but sometimes the host's metabolism causes limitations, so the modification of the host organism itself is preferable. Genetic engineering of strains is a common tool to enhance process productivity and overall efficiency. But even in the days of sequencing, not all production strains are fully sequenced, as, unfortunately, knowledge of underlying genes is a basic condition for genetic engineering. Another method for genetic modification, not as directed and specific as genetic engineering but also very effective, is adaptive evolution. By continuous environmental changes through enhancement of a stressor concentration or intensity and a following selection, cells can be adapted. An advantage of the so-called adaptive laboratory evolution (ALE) is that the change of environment can happen in a fast and flexible way[16−18]. The whole organism with all its functions can be adapted to certain environmental conditions, not just a single gene. Successful adaptation experiments paired with a following genomic or transcriptomic analysis can additionally lead to enhanced knowledge about underlying genes or gene regulation, enabling later targeted modifications[19,20]. The big challenge of this method is that it is random[21−23]. One can add a stressor to the medium and increase it regularly, but at the same time, the organism adapts to other growth conditions in which the adaptation takes place, which could lead to problems when the adapted variant is transferred to a different cultivation system than it was used in, like a BES[24]. For most cultivation conditions, this does not seem to be an issue that requires immediate innovative solving, as there often can be a quick fix by just changing the cultivation method during ALE. However, there is no such solution for electroactive cultivation conditions. Standard cultivations in BES usually take several days, in addition to its preparation. The common way of adaptation, regularly transferring culture to fresh medium in intervals and increasing the concentration of the stressor gradually, is not applicable here[12,20,25]. Therefore, with an electrified Pioreactor®, the need for an electrochemical adaptive laboratory evolution (eALE) platform could be realized. The aim of this study was the electrification of the Pioreactor® for two different electrobiotechnological applications with different setups. The first setup was built for a common usage of the production host C. necator in BES: the indirect electron transfer via H2 that is electrochemically produced by water splitting in a two-electrode, one-chamber setup and aeration with CO2 and O2[15]. The second setup was constructed for the newly discovered BES application with C. necator and its use for anodic respiration via MET[13].
-
The cultivation of all C. necator strains was started from a cryo-conserved stock culture stored at −80 °C. Cells were spread on an LB agar plate (5 g/L NaCl, 5 g/L yeast extract, 10 g/L tryptone, 1.8% agar, pH 7) and incubated at 30 °C for 24–48 h. Five millilitres of LB medium (5 g/L NaCl, 5 g/L yeast extract, 10 g/L tryptone, pH 7) were inoculated from a single colony and incubated in an orbital shaker overnight[26]. All liquid cultures of C. necator were incubated at 30 °C and shaken at 180 r/min (Multitron II, Infors AG, Bottmingen, Switzerland). Cells from the LB-preculture were harvested by centrifugation (14,000 r/min, 10 min, Centrifuge 5417C, Eppendorf, Germany) and subsequently washed twice in minimal medium containing 4 g/L fructose following an established protocol[27]. The following minimal medium preculture was inoculated to an OD600 of 0.1 and cultivated for 24 h at 30 °C and 180 r/min. For heterotrophic cultivation, no further precultures were needed; the main culture in minimal medium with 4–20 g/L of fructose as a carbon source was inoculated to an OD600 of 0.1. For electro-autotrophic cultivation, precultures were prepared following an established procedure[15,27]: cells were harvested by centrifugation (4,700 r/min, 10 min) and washed twice in carbon-source-free minimal medium. The OD600 was then adjusted to 0.2, after which 25 mL of culture was transferred to a sterilized, gas-tight 250 mL flask and supplied with a 1 bar atmosphere of H2, CO2, and O2 (8:1:1). The sealed flasks were incubated at 30 °C at 180 r/min for 36 h. These autotrophic precultures were harvested and centrifuged at 4,700 r/min for 10 min at room temperature. The cells were used to inoculate the BES at an OD600 of 0.2.
For chemo-organic electro-fermentation of C. necator via MET[10] the heterotrophic minimal medium preculture was grown for 48 h to reach the stationary growth phase, following the previously reported approach[13]. The cells were harvested, washed, and resuspended in medium containing a redox mediator; in this case, 5 mM ferricyanide (FEC), at an OD600 of 2. All strains that were used in this study are listed in Table 1.
Table 1. List of strains used in this study.
Bio electrochemical systems – BES
Standard BES for electro-autotrophic cultivation
-
A standard BES was composed of an undivided electrochemical reactor with a working volume of 110 mL and a two-electrode setup derived from Langsdorf et al. and Sydow et al.[15,27]. Platinized titanium expanded metal with a surface factor of 1.7 (50 g Pt per m2, Metakem GmbH, Usingen, Germany) and a geometrical surface area of 6 cm2 was used as an anode for water splitting, and a graphite rod with a geometrical surface area of 6.48 cm2 was chosen as a cathode for the electrochemical production of H2. Both electrodes were contacted with a platinum wire with a diameter of 0.5 mm. The contact of the graphite rod was additionally secured with Teflon tape. The electrodes were held at a distance of 1 cm with a 3D-printed separator, printed with a heat-resistant polyamide fiber (Fiberthree F3 PA-GF30 Pro, Fiberthree, Darmstadt, Hessen, Germany) in the Prusa 3D-printer (Original Prusa i3 MK3S+ printer, Prusa Research a.s., Holešovice, Czech Republic). A current of 15 mA was applied constantly for water electrolysis via a potentiostat (Gamry Interface 1010B, Gamry Instruments, Warminster, PA, USA). For gas supply, PTFE tubing was mounted to the lid. For mixing at 300 r/min, a stir bar was added to the reactor. After autoclaving, the reactors were filled to a total volume of 110 mL with sterilized autotrophic minimal medium and prepared as previously established. Sterilized PTFE tubes were connected to autoclaved silicone tubes and sterile filters for a continuous gas supply consisting of N2, O2, and CO2 (85:5:10) at a flow rate of 25 mL/min. The reactors were placed in an incubator at 30 °C (TH 30, Edmund Bühler GmbH, Bodelshausen, Germany) and, after polarization under the given conditions overnight, were inoculated. To transfer the same setup to a smaller reactor system, the Pioreactor® (Pioreactor 20 mL v1.1, Waterloo, Canada)[9] was altered as follows: to insert electrodes, a customized screw cap was 3D-printed with a heat-resistant polyamide fiber (Fiberthree F3 PA-GF30 Pro) in the Prusa 3D-printer i3 MK3S+. The cap had a middle opening for a septum for maximal flexibility regarding the placement of PTFE tubes and electrodes. The electrodes were the same materials as described earlier, only reduced in size to fit the reactor. The anode was built from platinized titanium expanded metal with a surface factor of 1.7 (50 g Pt per m2, Metakem GmbH, Usingen, Germany) and a geometrical surface area of 0.6 cm2, and a graphite rod with a geometrical surface area of 0.61 cm2 was used as a cathode. Therefore, the ratio of electrode surface per volume (working volume) is reduced in the one-chamber electrified Pioreactor® (0.07 cm2/mL) compared to the initial reactor setup (0.11 cm2/mL). For the reactions at the electrodes, a current of 3 mA was applied with a potentiostat (Gamry Interface 1010B, Gamry Instruments, Warminster, PA, USA). The resulting current density is enhanced in the one-chamber electrified Pioreactor® (4.5 mA/cm2) compared to the initial reactor setup (1.2 mA/cm2). The Pioreactor® stirs at 500 r/min with a magnetic stirrer and a stir bar and heats with a heating pad to 30 °C. Additionally, the whole reactor setup was placed in an incubation hood (TH 30, Edmund Bühler GmbH, Bodelshausen, Germany) to ensure the medium reservoir used for continuous experiments was preheated. Growth was measured via OD600 over a set of photodiodes in the lower region of the reactor. The peristaltic pumps, photodiodes, magnetic stirrer, and heating pad were controlled over a Raspberry Pi with an online interface. Two peristaltic pumps that come with silicone tubing were used to pump in and out of the 20 mL vessel for continuous experiments. After sterilizing the reactor by autoclaving, they were filled with 15–18 mL of sterilized autotrophic minimal medium depending on the operating mode. Sterilized PTFE tubes were connected to autoclaved silicone tubes and sterile filters for a continuous gas supply consisting of N2, O2, and CO2 (85:5:10, % [v/v]) at a flow rate of 25 mL/min. After polarization under the given conditions overnight, the reactors were inoculated. A scheme and a photo of the setup is shown in Fig. 1.
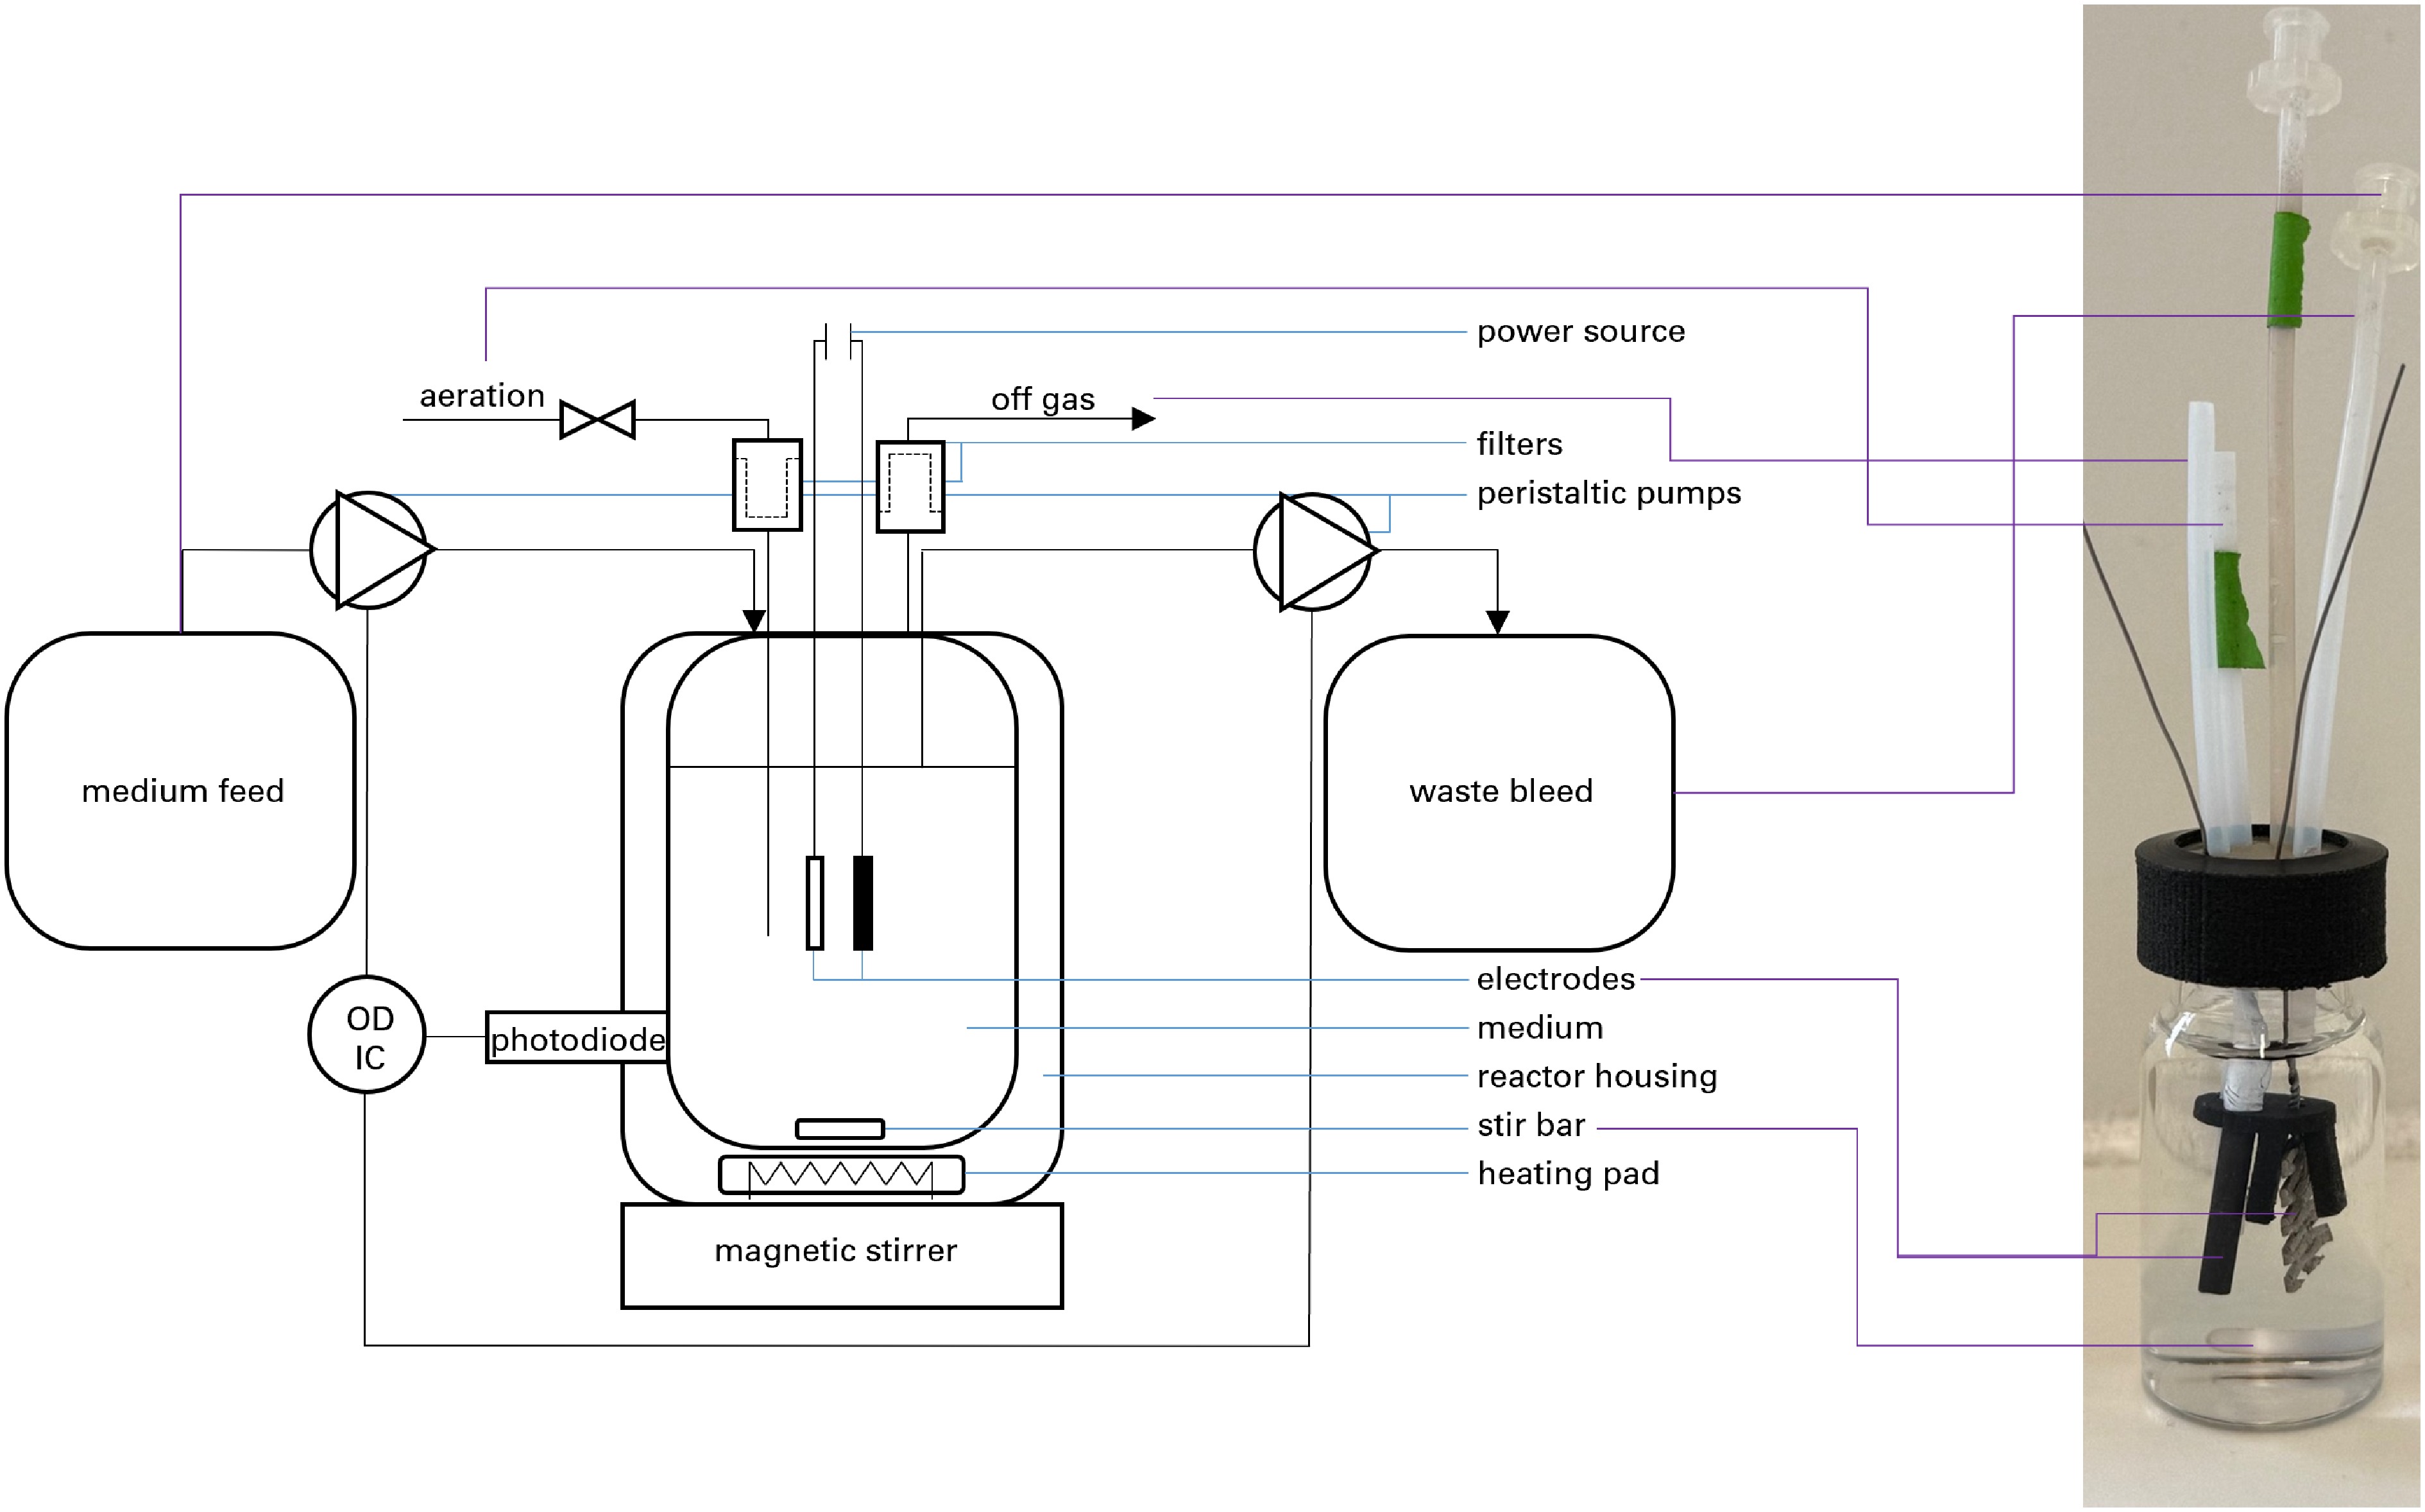
Figure 1.
Scheme and photo of the electrified Pioreactor® in a two-electrode one-chamber configuration with optional feed and bleed appliance.
Electrochemical adaptive laboratory evolution - eALE
-
For adaptation under electro-autotrophic conditions, the same precultures and setup were used as for electro-autotrophic cultivation with the Pioreactor®. Two peristaltic pumps were used to pump medium into the 20 mL vessel and to pump culture broth out of it. In turbidostatic mode, the desired OD600 was set in the user interface of the reactor. As soon as the culture reached it, the desired OD600 was kept stable by the addition of medium and discarding waste with the pumps. This cycle was repeated as long as it took to dilute the growing culture. For adaptation during electro-autotrophic cultivation, the feed media was supplemented with 350 mM Na2SO4 to a higher osmotic pressure. A scheme and a photo of the setup is shown in Fig. 1.
BES for chemo-organotrophic electro-fermentation
-
The main vessel of the reactor, a 20 mL glass vial, was the anodic chamber and was filled with the medium according to Sydow et al[27]. The cells are commonly cultured with 20 g/L fructose as a carbon source. It was further supplemented as described before with 5 mM FEC to enable MET. The cap had a middle opening for a septum for maximal flexibility regarding the placement of tubes, the second chamber, and electrodes. As an anode, a graphite rod with a geometrical surface of 0.61 cm2 was used. The cathode was built from platinized titanium expanded metal (50 g Pt per m2, Metakem GmbH, Usingen, Germany) with a geometrical surface area of 1.07 cm2. Both electrodes were connected with a titanium wire with a 0.5 mm diameter to the graphite rod. It was additionally fixed with Teflon tape. The cathodic chamber was built from a shortened Luggin capillary with a thread at the top to seal it with a screwcap and a pierceable septum for a gas-tight connection. The cathode buffer was composed as derived from the sodium phosphate buffer of the used minimal medium with Na2HPO4/NaH2PO4, supplemented with 150 mM Na2SO4. According to the formal potential of the mediator, a potential of 500 mV vs. the reference electrode was applied, as shown in Gemünde et al.[13]. As the reference electrode, the 11 cm low-profile Ag/AgCl electrode from Pine Research was used (Pine Research, North Carolina, USA). Consistent with the setup described above, the Pioreactor® was agitated with a magnetic stirrer at 500 r/min and maintained at 30 °C using its integrated heating pad. Additionally, the whole setup was placed in an incubation hood, so extended features like the cathode chamber were kept at the desired temperature (Fig. 2).
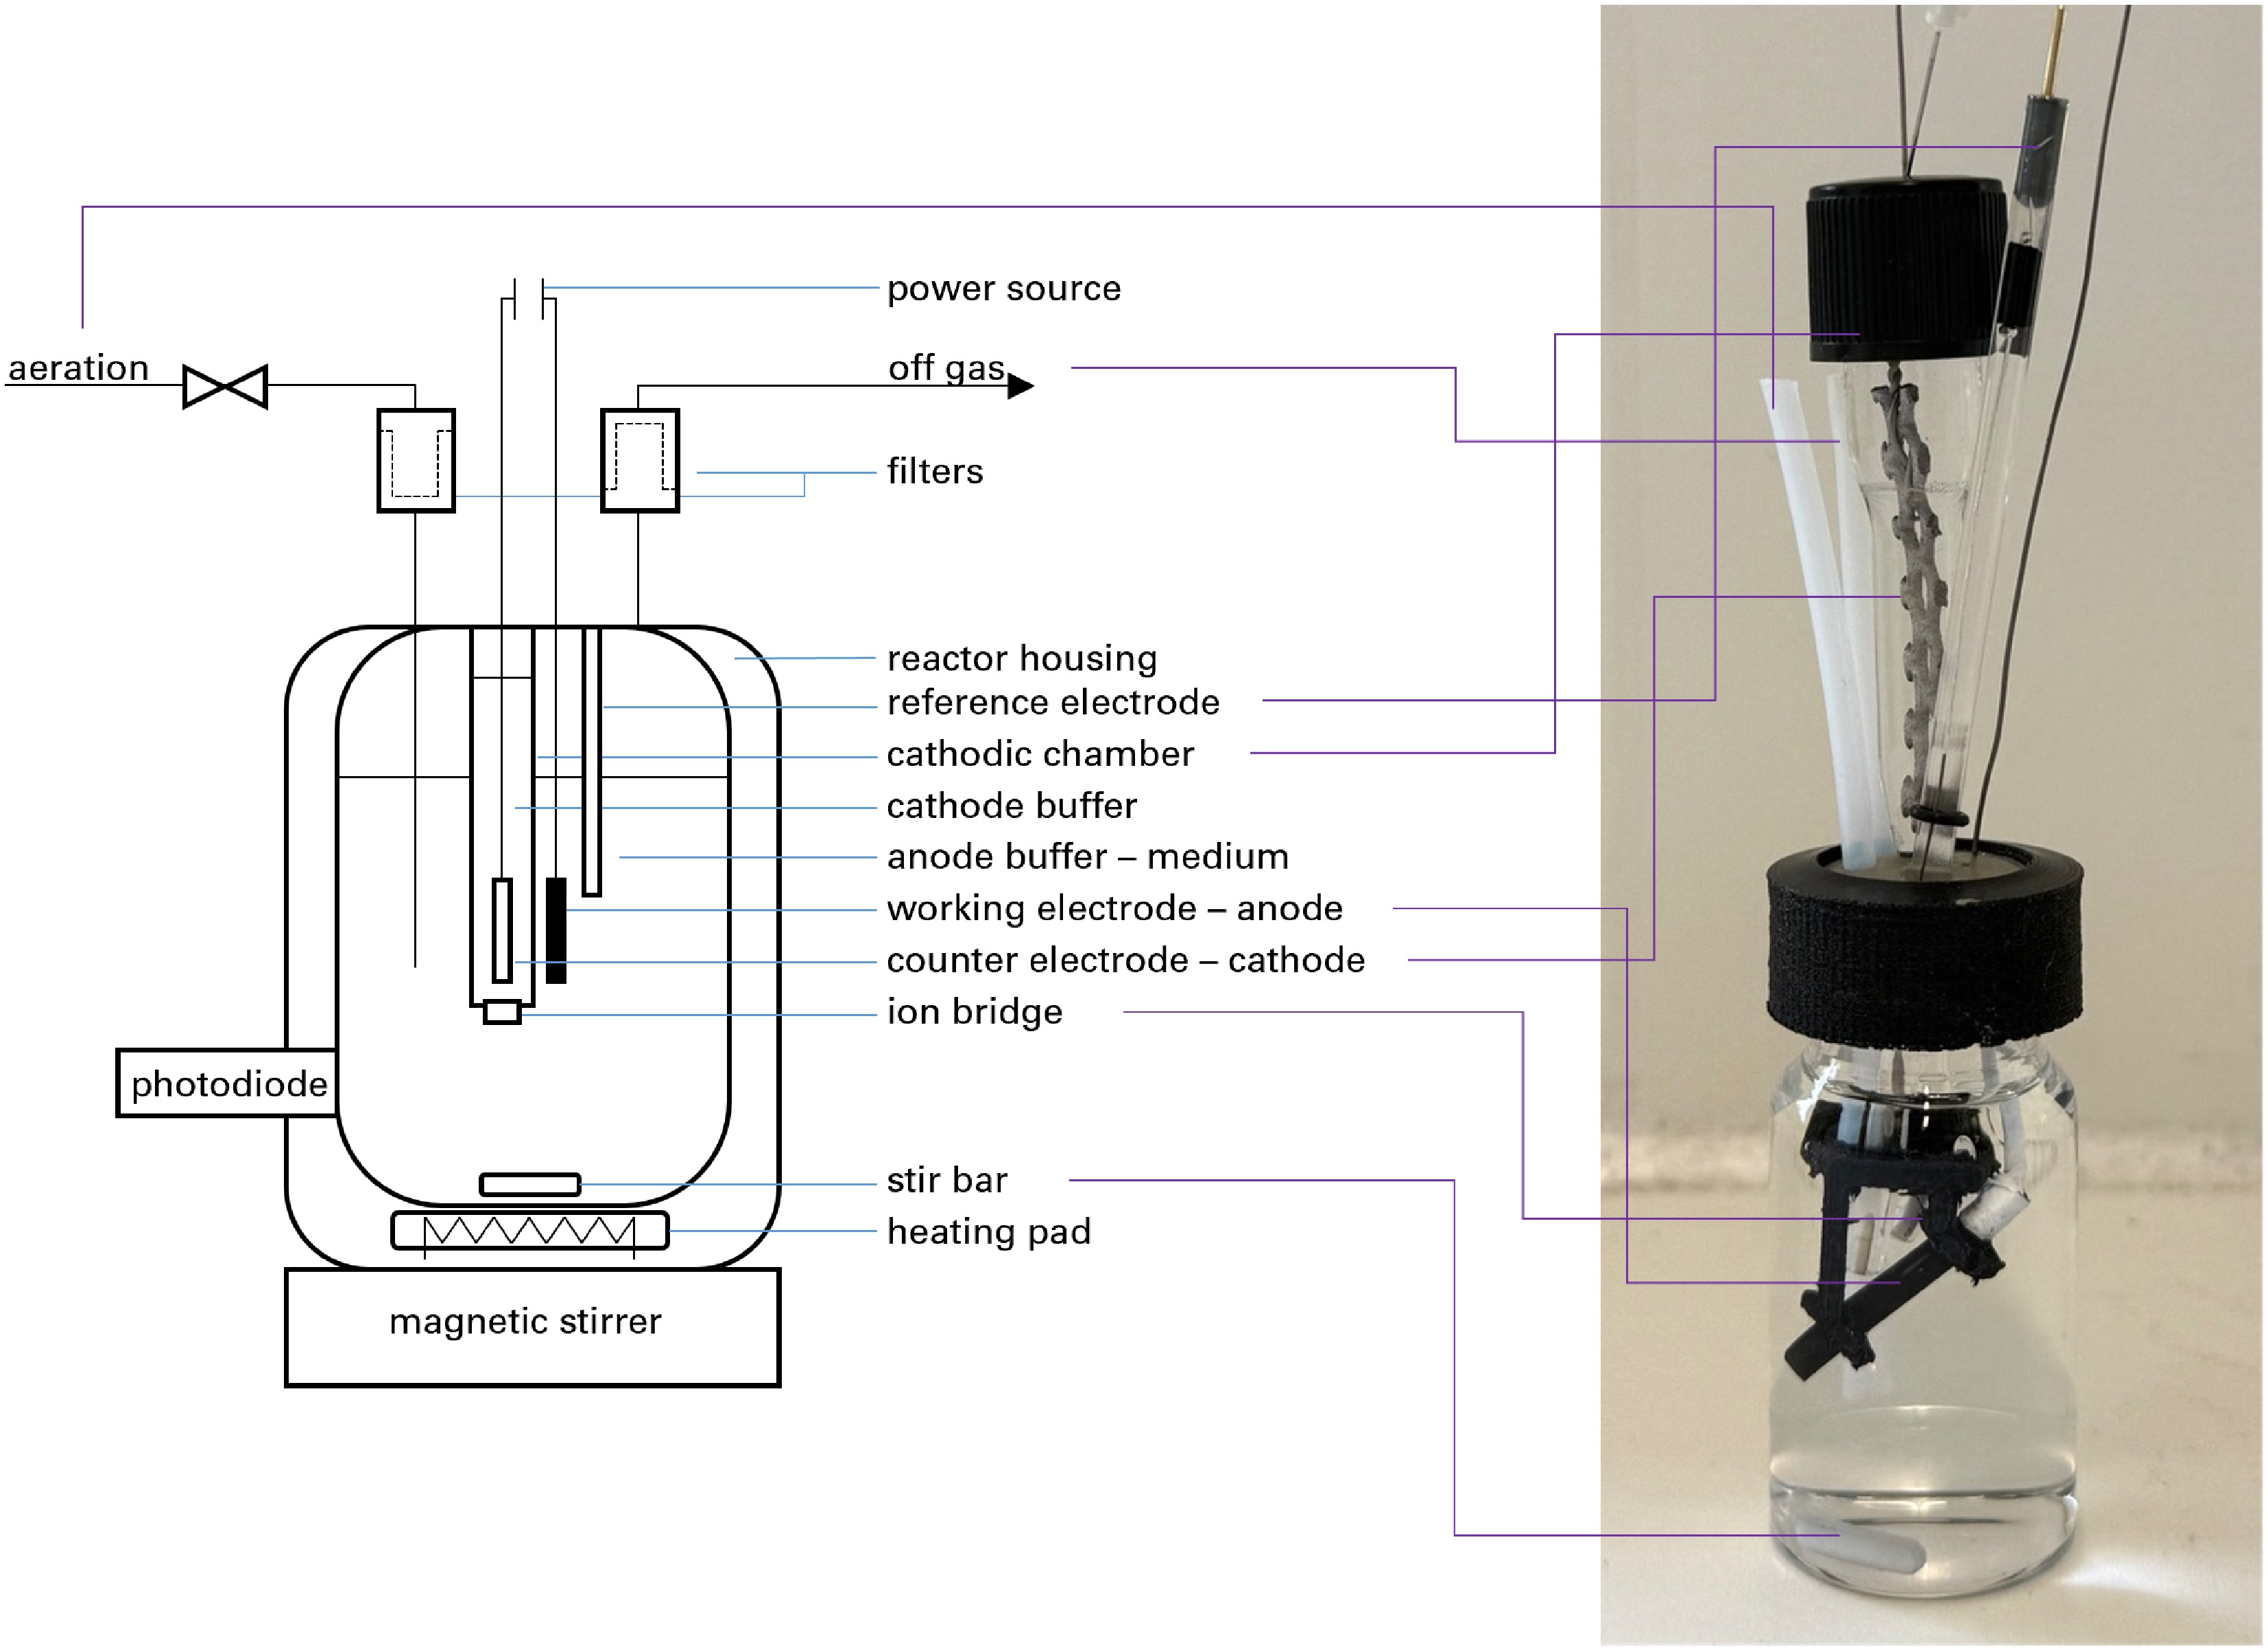
Figure 2.
Scheme and photo of the electrified Pioreactor® in a three-electrode two-chamber configuration.
Analytics
Growth analytics
-
Growth was measured photometrically via the optical density of culture samples or diluted samples at a wavelength of 600 nm (OD600) in a tabletop photometer (Genesys 30, Thermo Fisher Scientific Inc., USA) as well as the Stratus microplate reader (Cerillo, Charlottesville, VA, USA). Kinetic measurement of growth in the microplate reader was performed at 30 °C at 500 r/min on a Thermomixer C (Eppendorf, Germany). During eALE, the optical density was measured with the Pioreactor®-integrated photodiodes. The photodiodes were calibrated beforehand according to the manufacturer's instructions; they were able to measure optical density at a wavelength of 600 nm up to a value of 2.5. The dilution rate in the continuous cultivation was calculated according to Eq. (1) with the mean value of the feed volume. The Na2SO4 concentration over time during the continuous eALE process was estimated via Eq. (2) with an initial concentration of 0 mM Na2SO4 and 350 mM Na2SO4 in the feed medium. Growth rates were calculated via Eq. (3).
$ D (t) = \dfrac{\mathrm{F}(\mathrm{t})}{\mathrm{V}0}\;\;{\rm{ with}}\;\; F (t) = \dfrac{{\text{∆V}}_{Feed}}{\text{∆t}} $ (1) $ {\mathrm{c}}_{\mathrm{i}+1}={\mathrm{c}}_{\mathrm{i}}+\dfrac{{\Delta \mathrm{V}}_{\mathrm{i}}}{\text{VR}}({\mathrm{c}}_{\text{Feed}}-{\mathrm{c}}_{\mathrm{i}}) $ (2) $ {\text{µ}} =\dfrac{\Delta{\text{(lnOD}}_{600})}{\Delta\text{t}} $ (3) Redox-state, pH
-
The redox state of the mediator ferricyanide was measured at a wavelength of 420 nm in the above-mentioned photometer. pH was measured at single timestamps during cultivation with a pH meter (pH-meter Lab 845, SI Analytics–Xylem Analytics Germany, Mainz, Germany).
Gas and sugar analytics
-
The composition of the gas phase was controlled daily using a gas analyzer (Gas Analyser Micro GC Fusion, Inficon Holding AG, Bad Ragaz, Switzerland). The column used was the DB-WAX (30 m) with an inner diameter of 0.25 mm and a 0.25 µL film (Agilent Technologies GmbH, Waldbronn, Germany). Carrier gases were in channel A, argon, and in channel B, helium; the detector was a thermal conductivity detector (Inficon Holding AG, Bad Ragaz, Switzerland). A gas sample of 3 mL was manually inserted and measured for 2 min; the estimated retention times in seconds for carbon dioxide was 23.7, for hydrogen 48.4, for oxygen 59, and for nitrogen 67.4.
Consumption of fructose was measured via HPLC as described previously. Briefly, fructose was measured as adapted from Löwe et al. via HPLC (Agilent 1100 Series, Agilent Technologies, Santa Clara, CA, USA)[29]. As the mobile phase, 5 mM H2SO4 was used with a flow of 0.5 mL/min. The stationary phase was a Rezex ROA-Organic Acid H+ (8 %), LC Column 300 mm × 7.8 mm (Phenomenex, Aschaffenburg, Germany) with a Rezex ROA-Organic Acid H+ (8%), LC Column 50 mm × 7.8 mm used as a precolumn (Phenomenex, Aschaffenburg, Germany), and they were heated to 55 °C. For the detection of sugars, a refractive index detector (Agilent G7162A 60 Infinity II RID, Agilent Technologies, Santa Clara, CA, USA) was used and run at 55 °C. Samples of 10 µL were run for 20 min; the expected retention time of fructose was 14.7 min. Evaluation and analysis were performed with OpenLAB CDS software of Agilent (Agilent Technologies, Santa Clara, CA, USA). Samples were prepared by centrifuging in a tabletop centrifuge (Centrifuge 5417C, Eppendorf, Germany) at 14,000 r/min and room temperature for 10 min and filtering the supernatant with a syringe filter. A 100 µL sample was transferred into a glass vial with an insert and kept at 4 °C until analysis.
-
For a first test cultivation, C. necator H16ΔPHB was used in the electrified reactor in a one-chamber setup with two electrodes (Fig. 1). After overnight polarization with 3 mA and aeration with 25 mL/min with N2 : O2 : CO2 (85:5:10, % [v/v]), the BES was inoculated to an OD600 of 0.2. Instead of measuring the growth of the culture with the Pioreactors® own photodiodes, they were analyzed in a tabletop photometer. In the first 4–5 d of the cultivation shown in Supplementary Fig. S1, the growth of C. necator H16ΔPHB was linear, consistent with previous observations[15], before reaching an OD600 of about 8.5 and its maximum of around 9 at day 6, before decreasing again at day 7 to 8.5. The resulting OD was approximately two times higher than in a comparable investigation in modified Schott flasks[15]. This could be related to the enhanced current density in the one-chamber electrified Pioreactor®.
After this successful pre-experiment, in the one-chamber system electrified Pioreactor®, the peristaltic pumps were used for the turbidostatic cultivation. During the turbidostatic cultivation, the aim was to keep the optical density at 1. For the sake of adaptation, only the feed medium was supplemented with 350 mM sodium sulphate, so after every adjustment of OD600, the sodium sulphate concentration increased step-by-step. This way, over the duration of 10 d, the cells were steadily adapted to a higher salt concentration, which could result in an enhanced osmotolerance under electro-autotrophic cultivation conditions. In Fig. 3, the described adaptation process is shown. During eALE, C. necator H16ΔPHB was adapted over a period of only 10 d to enhanced sodium sulphate concentrations with a feed of minimal medium supplemented with 350 mM of sodium sulphate. After an initial growth phase of nearly 1 d, the desired OD600 of 1 was reached, and the feed was regulated by the turbidostatic settings. During the eALE, the voltage was a little higher; around inoculation, it lay at 3.1–3.2 V and decreased more strongly as the feed with the electrolytic sodium sulphate started after a day to around 2.7 V until the end of the cultivation. After 10 d, the total feed volume reached nearly 120 mL, with a working volume of 18 mL; that's 6.7 times the initial volume of the reactor. For further characterization, the dilution rate was calculated via Eq. (1) with the mean value of the feed volume. Per hour, 0.54 mL of the feed medium supplemented with 350 mM of Na2SO4 was added (12.96 mL per day), resulting in a dilution rate of 0.03 h−1. Additionally, with the feed volume and the known starting concentration of Na2SO4 as well as its concentration in the feed media (350 mM), the Na2SO4 concentration over time was calculated according to Eq. (2) (Supplementary Fig. S2). It's visible that after around 4–5 d of cultivation, already nearly 350 mM of Na2SO4 in the culture vessel is reached. Therefore, half of the adaptation time was spent in the final concentration of around 350 mM Na2SO4.
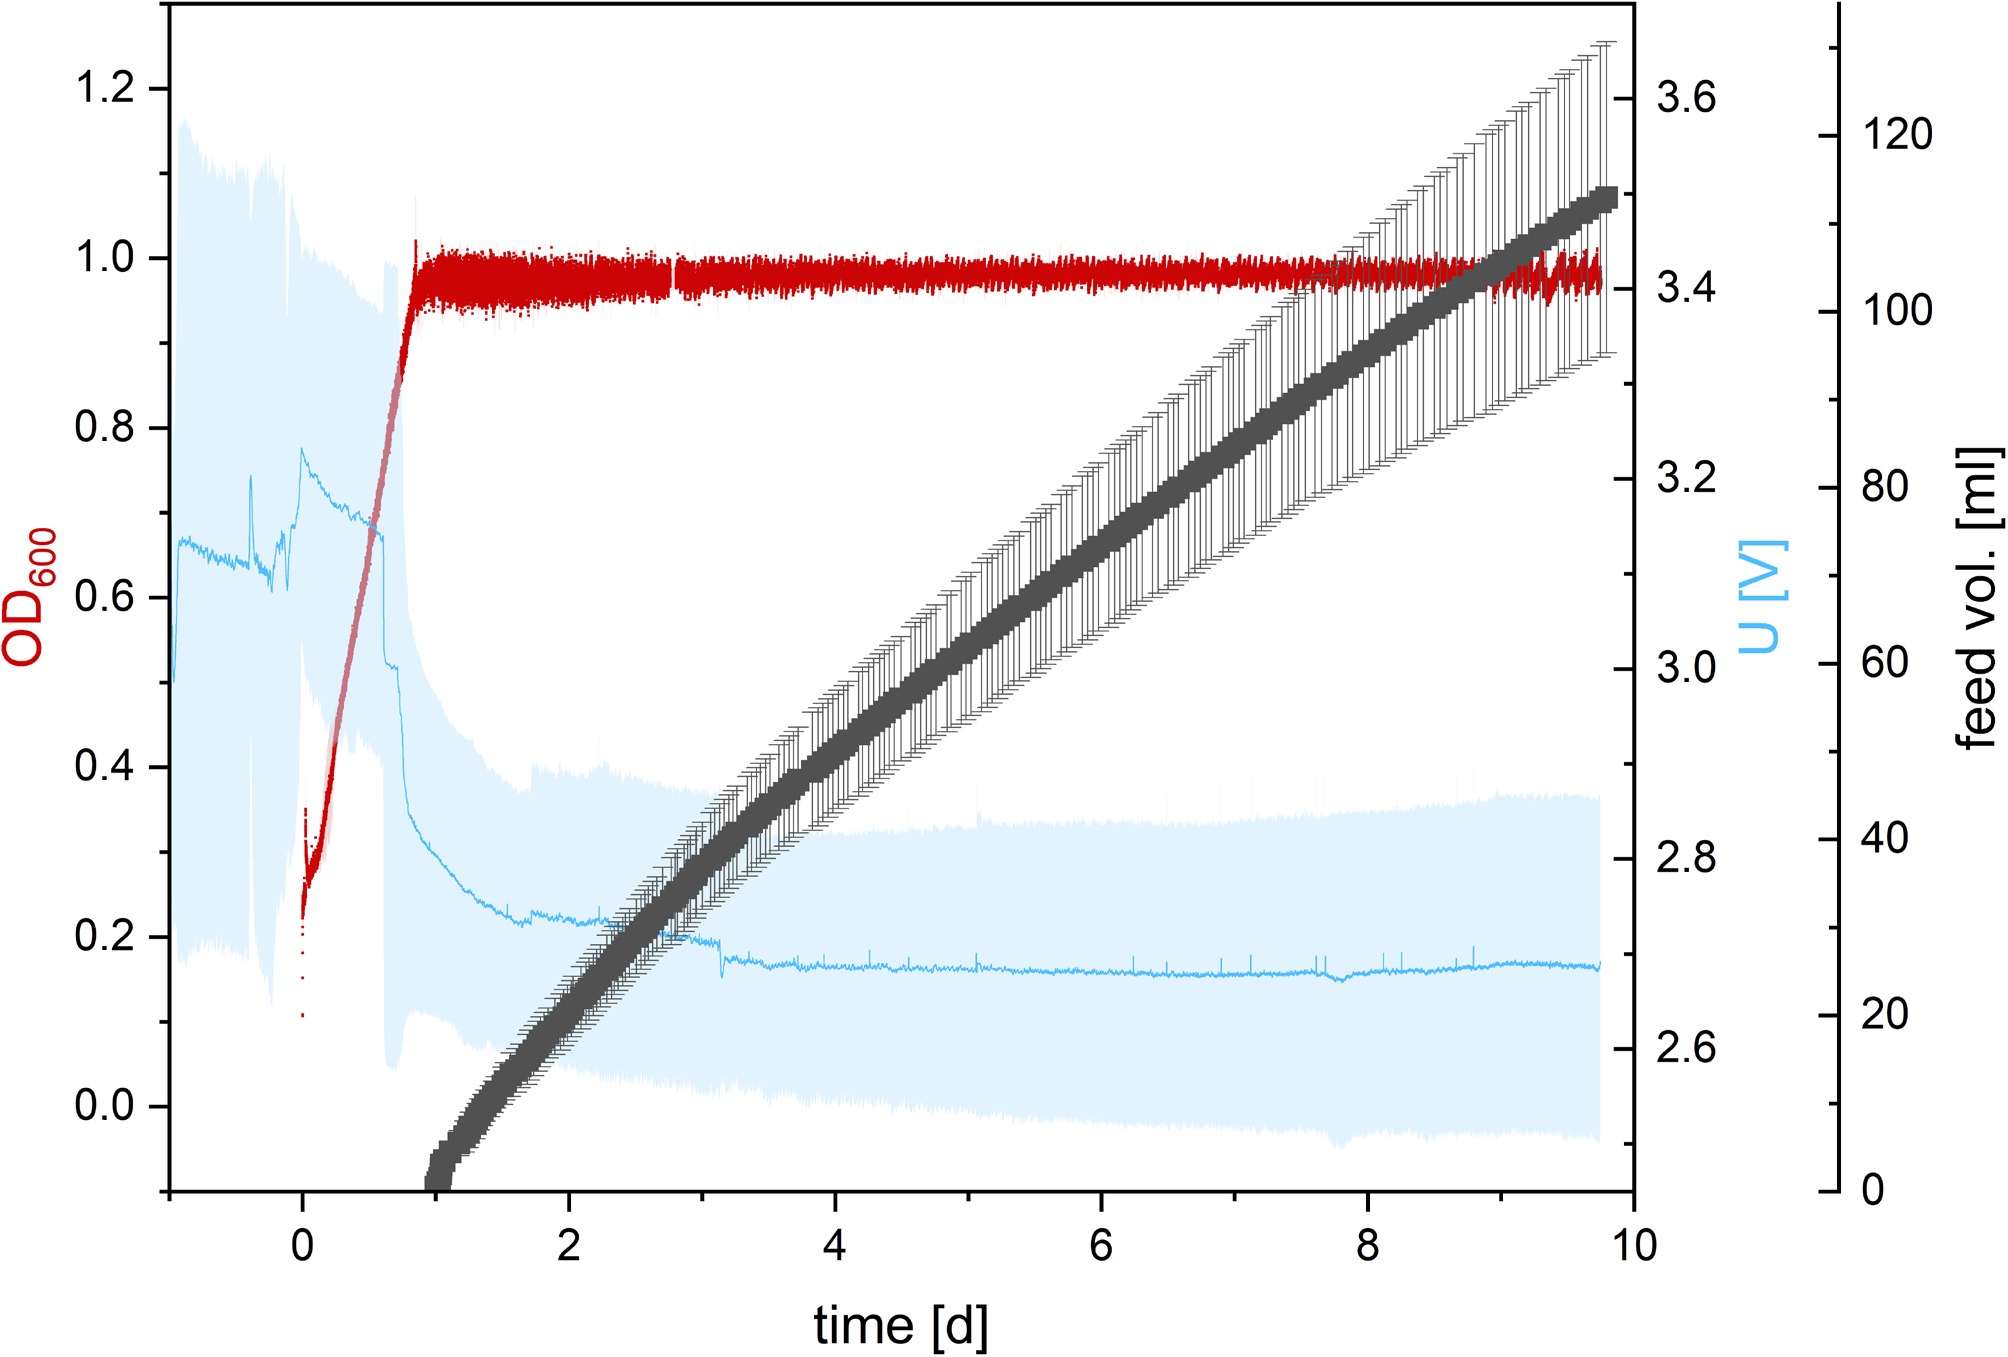
Figure 3.
Continuous cultivation in the two-electrode Pioreactor®. C. necator ΔPHB was cultivated in the electrified Pioreactor® under electro-autotrophic conditions in minimal medium at 30 °C and 500 r/min for 9 d. The reactors were supplied with a gas mixture of N2 : CO2 : O2 (85:10:5) at a flow rate of 30 mL/min. A current of 3 mA was applied for the water splitting reaction; the resulting voltage (blue) lay around 2.7 V after inoculation. The reactors were inoculated at an OD600 (red) of 0.2 and kept at 1 as soon as they reached it. The feed volume is shown as a black line (n = 2).
After the eALE, single colonies were isolated from the resulting culture. The strain was evaluated under heterotrophic conditions with different concentrations of sodium sulphate (Fig. 4). The adapted strain (red) was compared to the ΔPHB wildtype of the C. necator H16 strain (black) in minimal medium, supplemented with 0–500 mM sodium sulphate in the Stratus Cerillo microplate reader in a 96-well plate. During cultivation in minimal medium without any supplemented sodium sulphate, no difference between the two strains could be observed. On the contrary, it was visible that in medium supplemented particularly with 300 mM sodium sulphate, the adapted strain outperformed the wildtype. During the cultivation in 100 and 200 mM sodium sulphate medium, growth of the adapted variant already shows slightly better growth than the wildtype, which is visible in 300 mM medium even better, where the OD600 of the wildtype reached around 0.2–0.3 during the first 30 h of cultivation whereas the adapted strain had already reached 0.6 and continued growing stationarily to an OD600, max of 0.7 till the end of the cultivation of 48 h. The wildtype reached an OD600 of 0.55 after the total cultivation. During cultivation in medium supplemented with 400 and 500 mM sodium sulphate, no considerable growth was observed in either strain. The maximal specific growth rate between 6–20 h of cultivation was also calculated and statistically analyzed (Supplementary Table S1). Even though there are visible differences in growth, indicating that the adapted strain starts growing after a shorter lag phase and reaches a higher final OD600, the comparison of specific maximal growth rates during the exponential growth phase shows no statistically relevant differences.
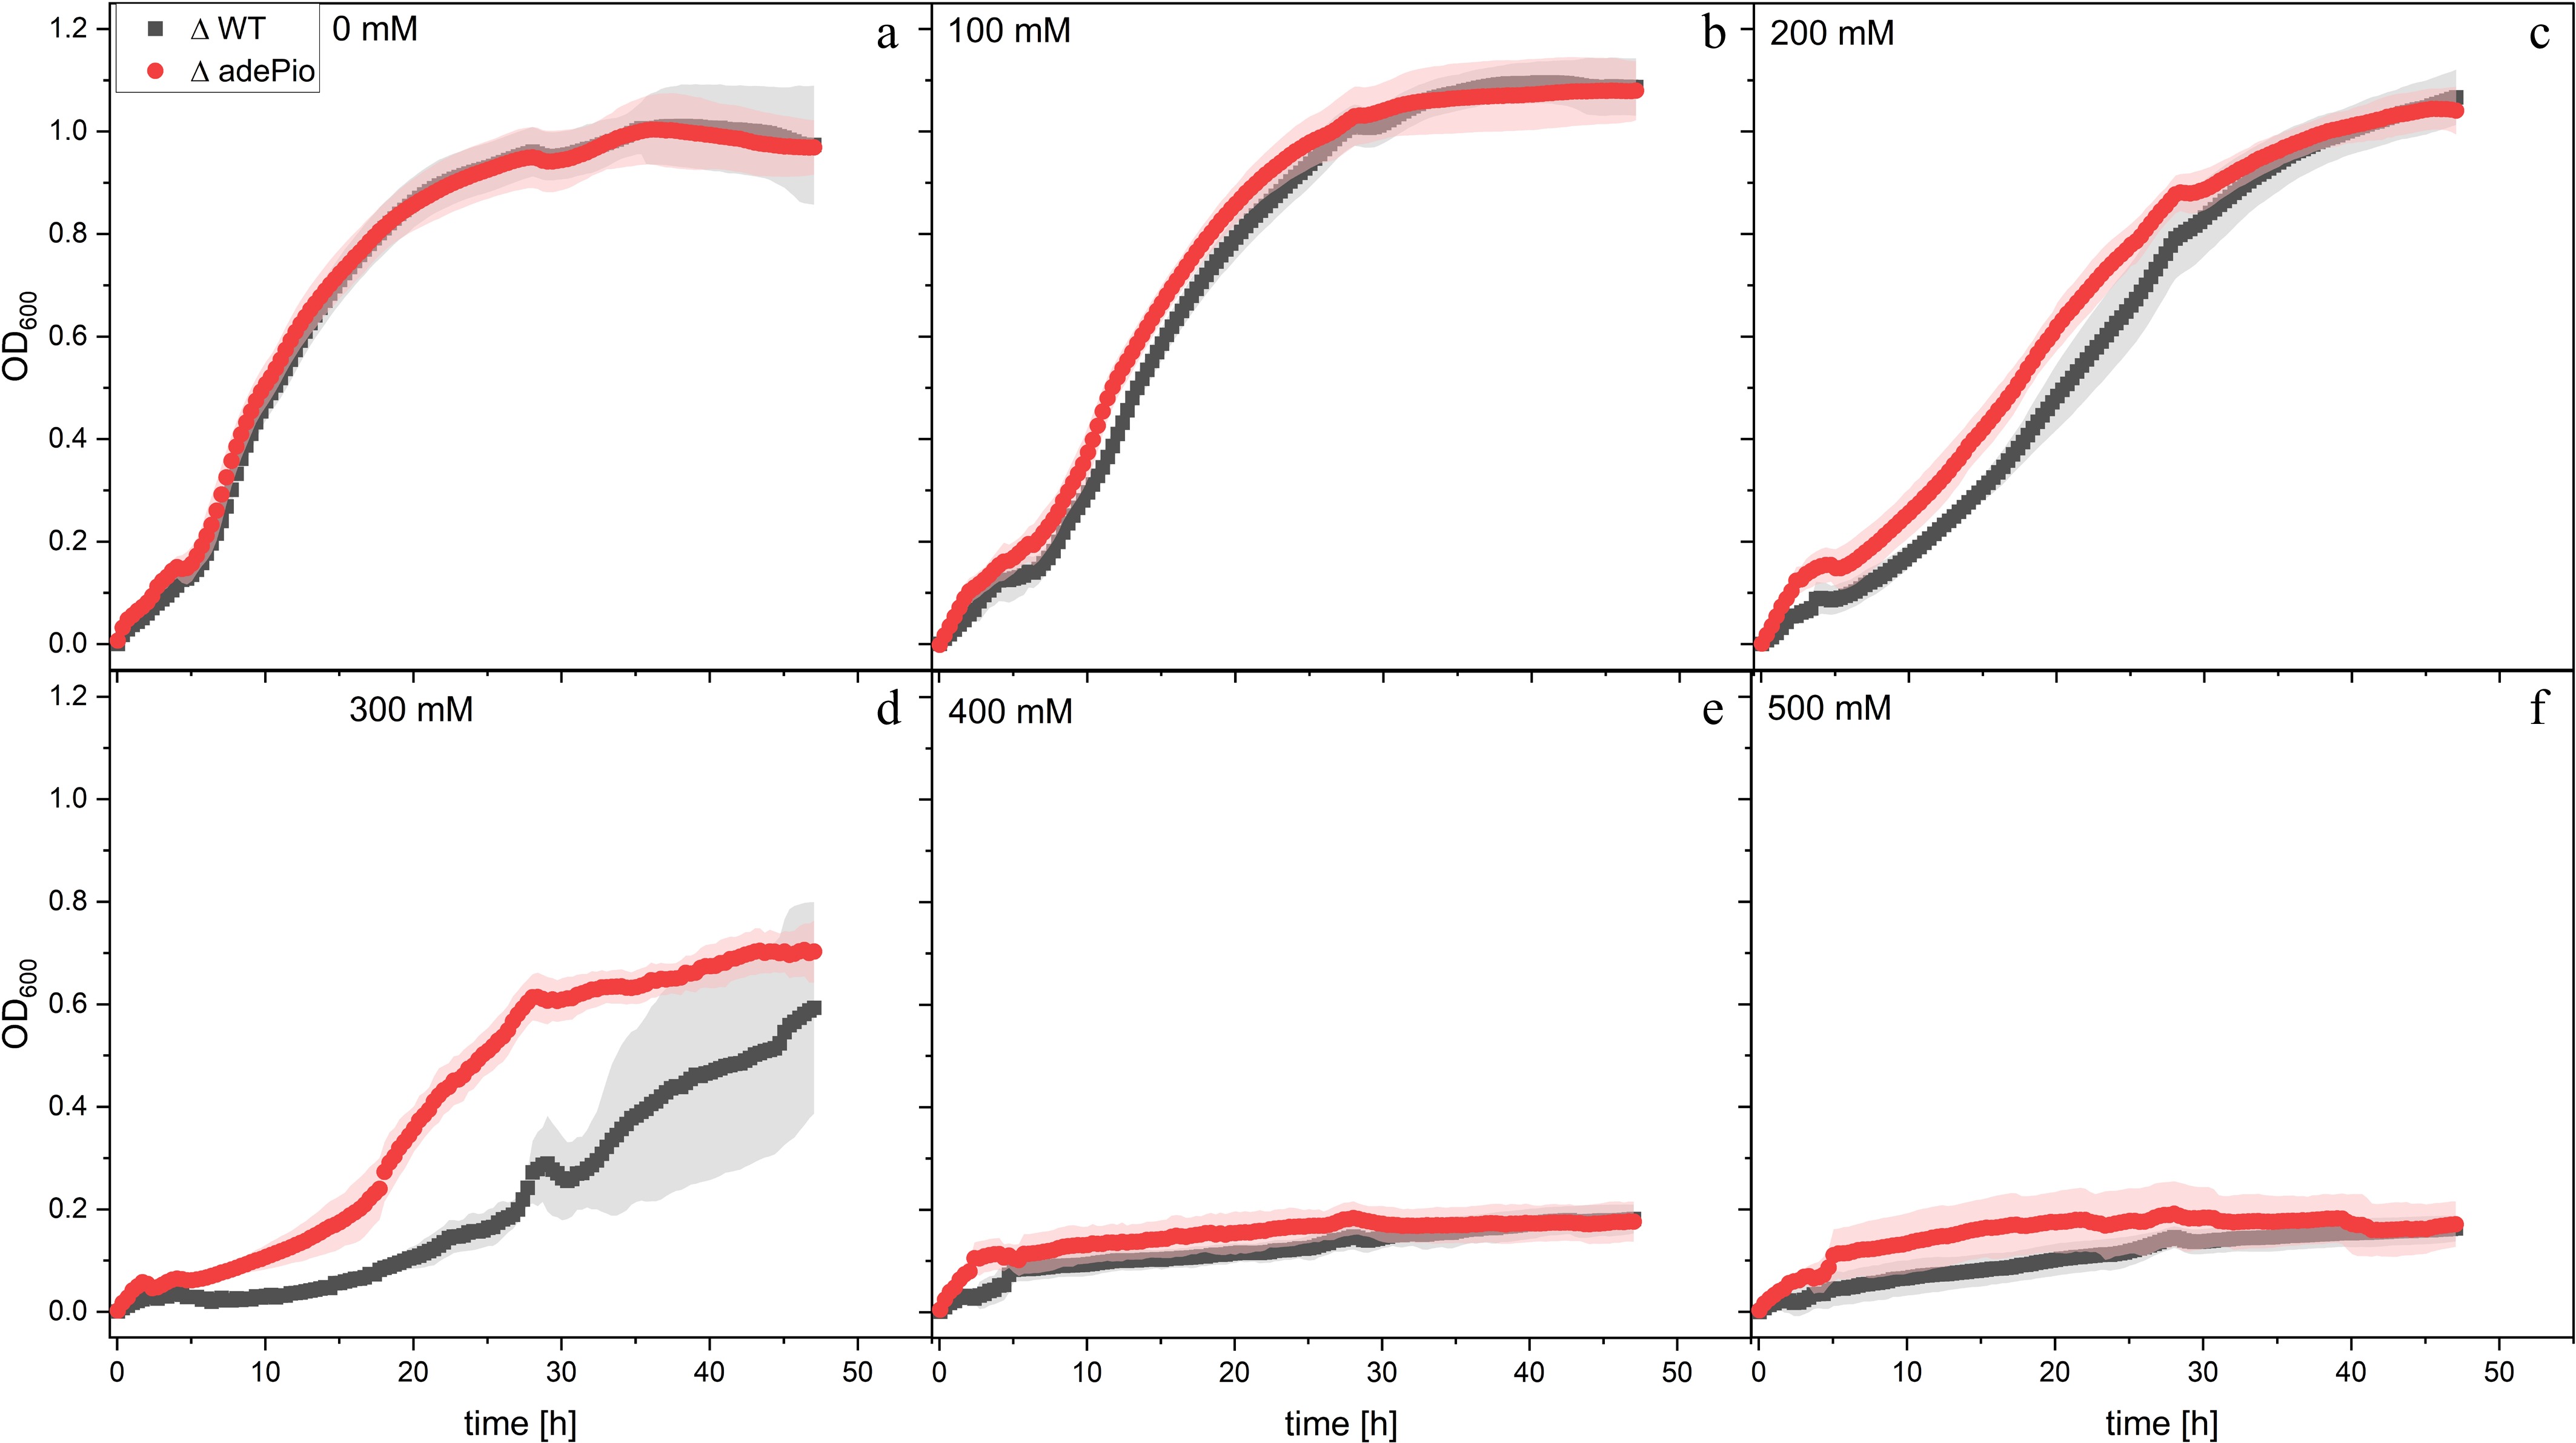
Figure 4.
Characterization under heterotrophic conditions of the Pioreactor® adapted C. necator ΔPHB adePio compared to the wild-type strain. C. necator ΔPHB (black) and C. necator ΔPHB adePio (red) were cultivated in a 96-well plate in the Stratus Cerillo microplate reader in minimal medium with (a) 0, (b) 100, (c) 200, (d) 300, (e) 400, and (f) 500 mM sodium sulphate at 30 °C and 500 r/min for 48 h, n = 6.
After the adapted strain showed better growth compared to the wildtype under heterotrophic conditions in minimal medium supplemented with 300 mM sodium sulphate, this concentration was chosen for an evaluation of the adapted strain under electro-autotrophic conditions. In order to investigate whether the eALE adaptation in 10 d could already have a permanent effect on growth under electro-autotrophic conditions, the adapted strain and the parental strain were grown in the original BES setup in a 110 mL reactor. As its final application in the 110 mL BES is the same, the resulting strain's performance can be benchmarked against a strain obtained via heterotrophic adaptation over a period of 60 d, which was characterized in an identical BES setup[21] despite the markedly different adaptation processes involved[30]. The reactors were polarized for 24 h at a current of 15 mA and aeration with the previously described gas mixture, before they were inoculated to an OD600 of 0.2 with autotrophic precultures. In this setup, the adapted strain also showed improved growth as indicated by OD600 compared to the wild-type strain (Fig. 5). Compared to the C. necator H16ΔPHB strain, which began to grow after 2 d, the adePio variant started growing after 1 d. After 6 d, the ΔPHB strain reached an OD600 of about 1.18 ± 0.12, whereas the adapted variant from the eALE process reached a higher OD600 of 1.57 ± 0.07. From this time on, the ΔPHB strain stagnated in growth. The adePio variant, on the other hand, grew further in the last days of cultivation to optical densities of around 2.69 ± 0.15. So, this leads to the consideration that even after a very short adaptational period in the electrified Pioreactor®, the eALE was successful, as it resulted in a strain that outgrew the original strain under heterotrophic and electro-autotrophic conditions while being under osmotic pressure through 300 mM sodium sulphate. Additionally, the growth rate of both strains was calculated from their average OD600 value according to Eq. (3). By the use of the turbidostatic mode, the adaptation could be more efficient, as the stressor concentration is enhanced as soon as the culture starts growing again. Even compared to classical ALE conducted in heterotrophic cultivation with the same stressor, where a resulting strain was adapted over a period of 60 d and afterwards transferred to BES where it was characterized under similar conditions as the herein adapted strain, the via eALE in 10 d adapted strain could keep up in performance reaching an OD600, max. of 2.69 ± 0.15 after 8 d, compared to an OD600, max of around 2.90 ± 0.09 after 216 h, equaling 9 d of cultivation of the classicaly adapted strain[30].
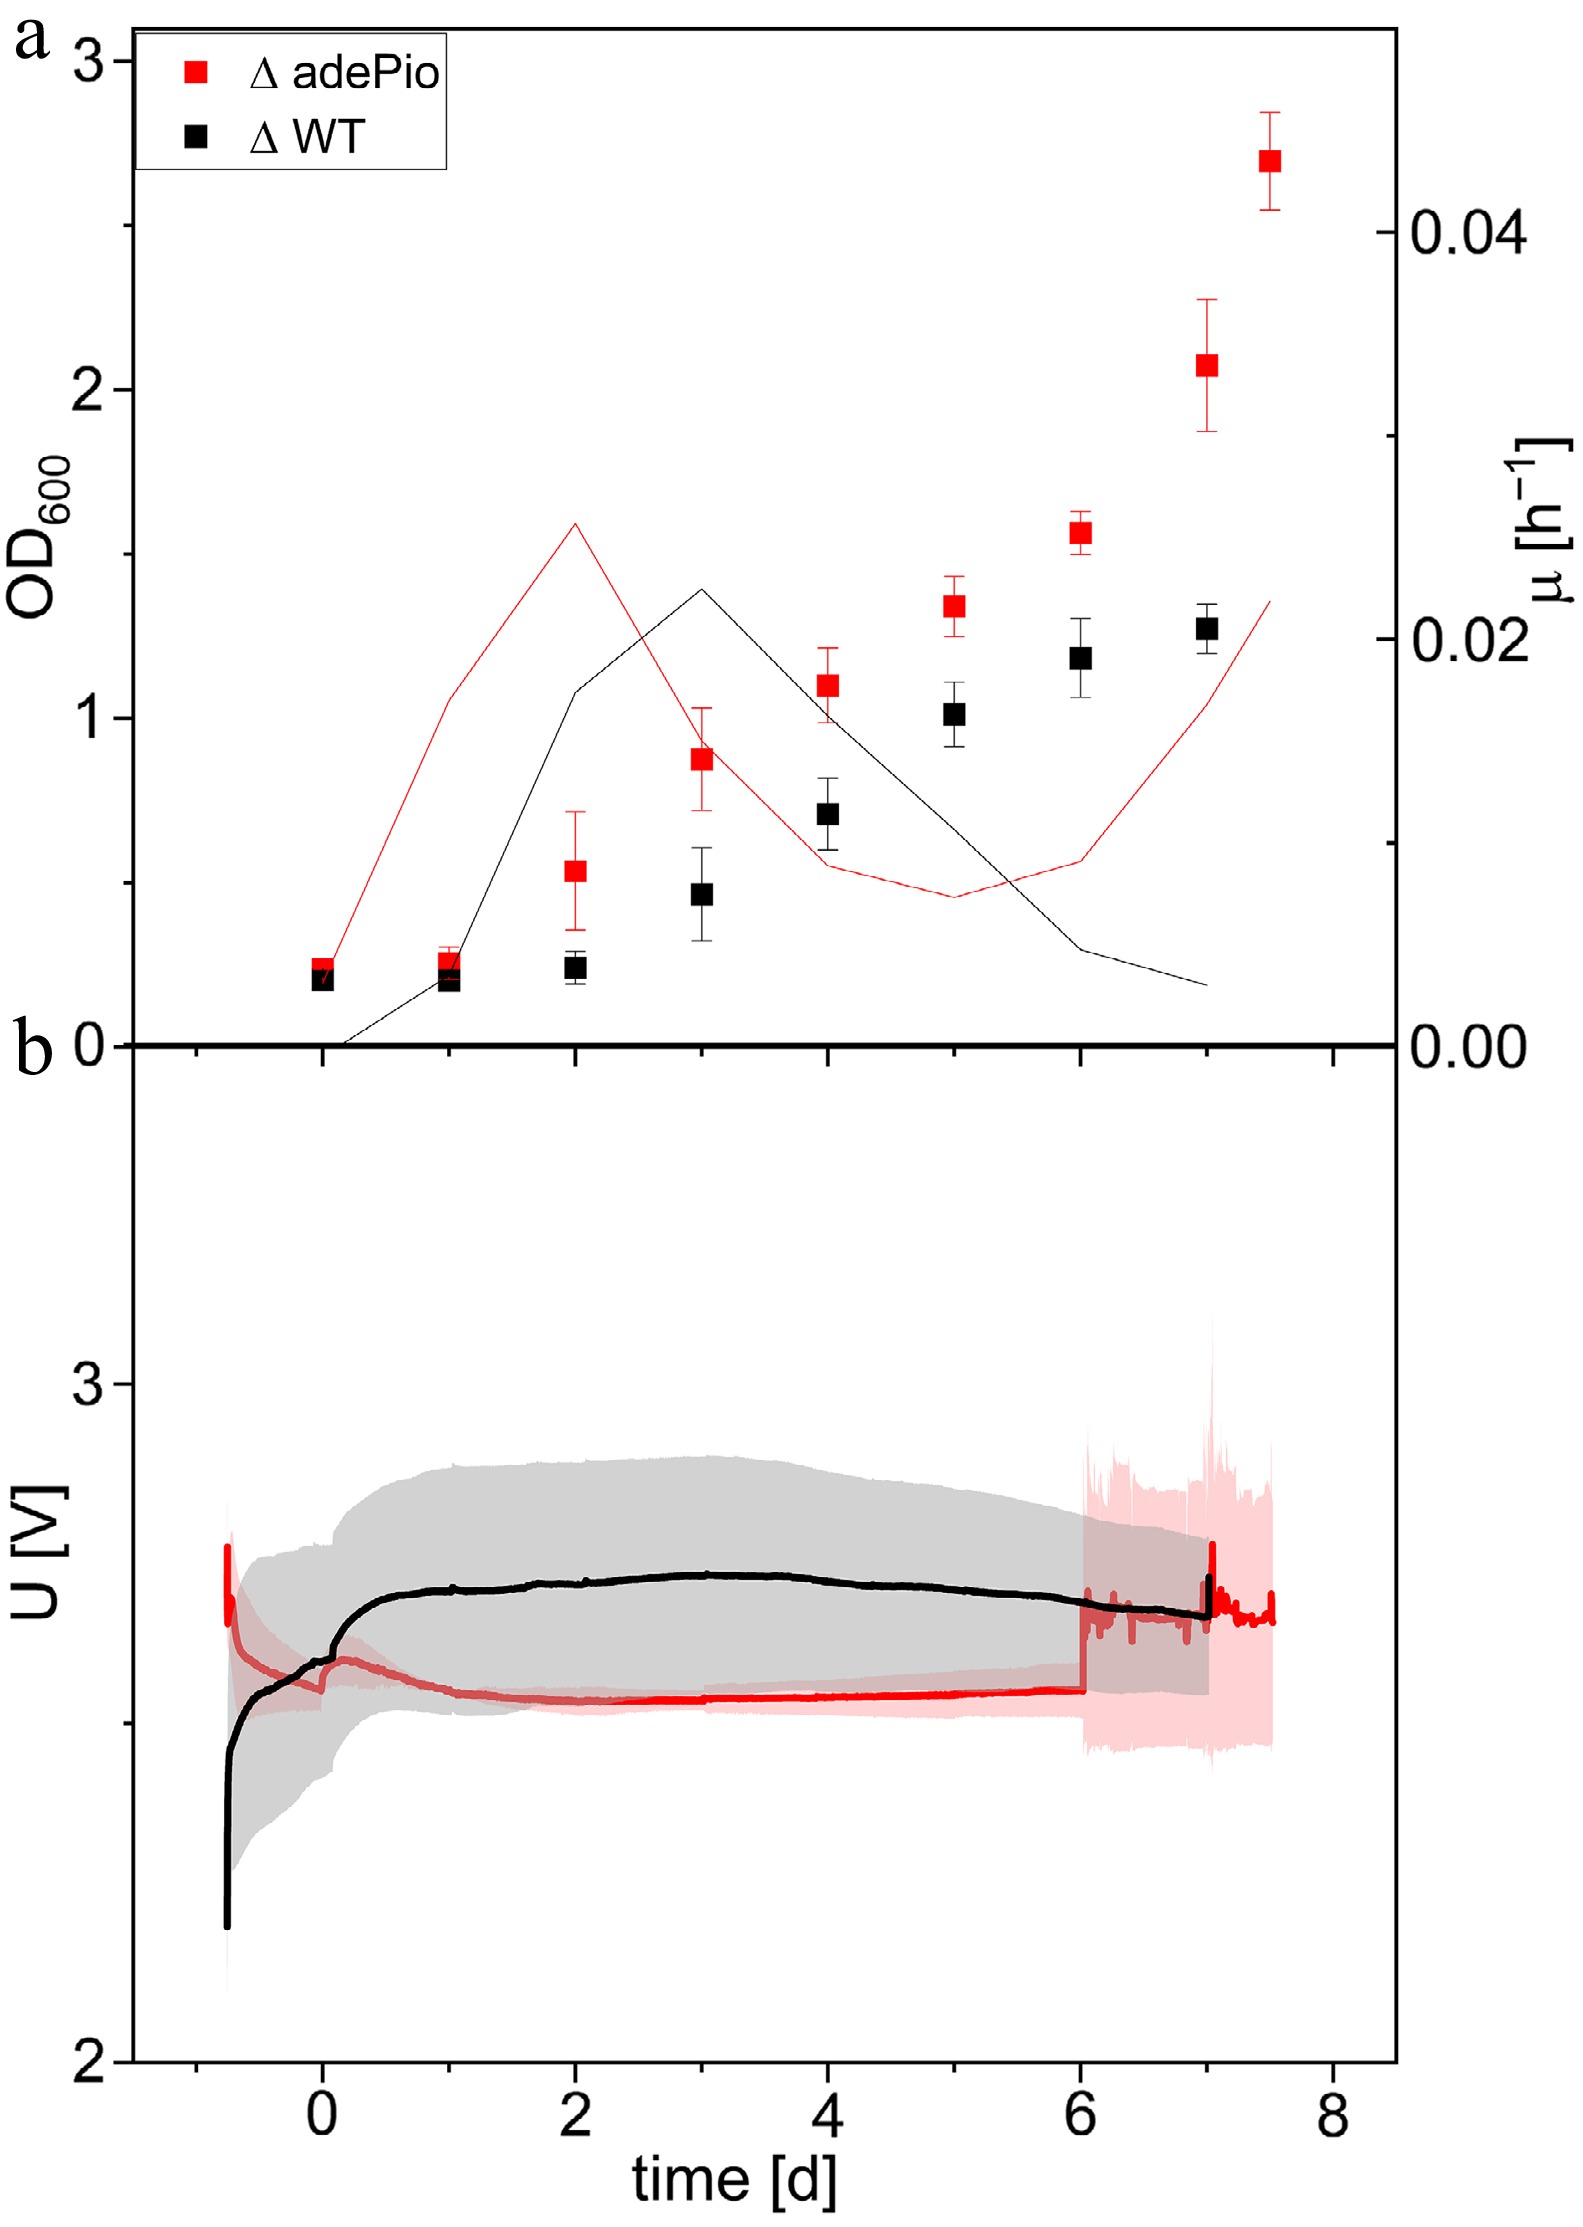
Figure 5.
Characterization under electro-autotrophic conditions of the Pioreactor® adapted C. necator ΔPHB adePio compared to the wild-type strain. C. necator ΔPHB (black) and C. necator ΔPHB adePio (red) were cultivated under electro-autotrophic conditions in minimal medium with 300 mM sodium sulphate at 30 °C and 300 r/min for 7.5 d. The reactors were supplied with a gas mixture of N2 : CO2 : O2 (85:10:5) at a flow rate of 25 mL/min. A current of 15 mA was applied for the water splitting reaction. Shown are the (a) OD600 and growth rate h−1, as well as (b) the measured voltage (n = 3).
To broaden the spectrum of possible use cases of the eALE platform that the electrified small-scale reactor offers, it was also electrified in another setup. A second chamber was added to the reactor by shortening a Luggin capillary with a ceramic frit fitted to the tip as an ion bridge and adding a thread so a screwcap with a septum could close the chamber. After polarization for 1 d, the reactors were inoculated with a stationary heterotrophic preculture to an OD600 of 1.75. As the medium was supplemented with 5 mM ferricyanide as a redox mediator, it was necessary to shield the reactor vial from light. This requirement was fulfilled by the housing of the reactor.
As shown in Fig. 6, the stationary culture of C. necator H16 stayed around the OD600 of inoculation (1.79 ± 0.07) during the cultivation before decreasing to 1.5 after 110 h. During the inoculation, the culture caused a peak current density of 550 µA/cm2 before it decreased to 175 µA/cm2 during the first 10 h of cultivation. The current density stayed steadily around 150–175 µA/cm2 for the next 85 h. After 100 h of cultivation, the current density decreased within 20 h to the level of the negative control around 0. Regarding the fructose consumption, the endpoint was analysed, resulting in a fructose value of 20.04 ± 1.41 g/L, indicating that no fructose was consumed, or just on a very low level, which might be overshadowed by evaporation due to gassing of the vessel, distorting the measurement. A comparable trend has previously been reported[13].
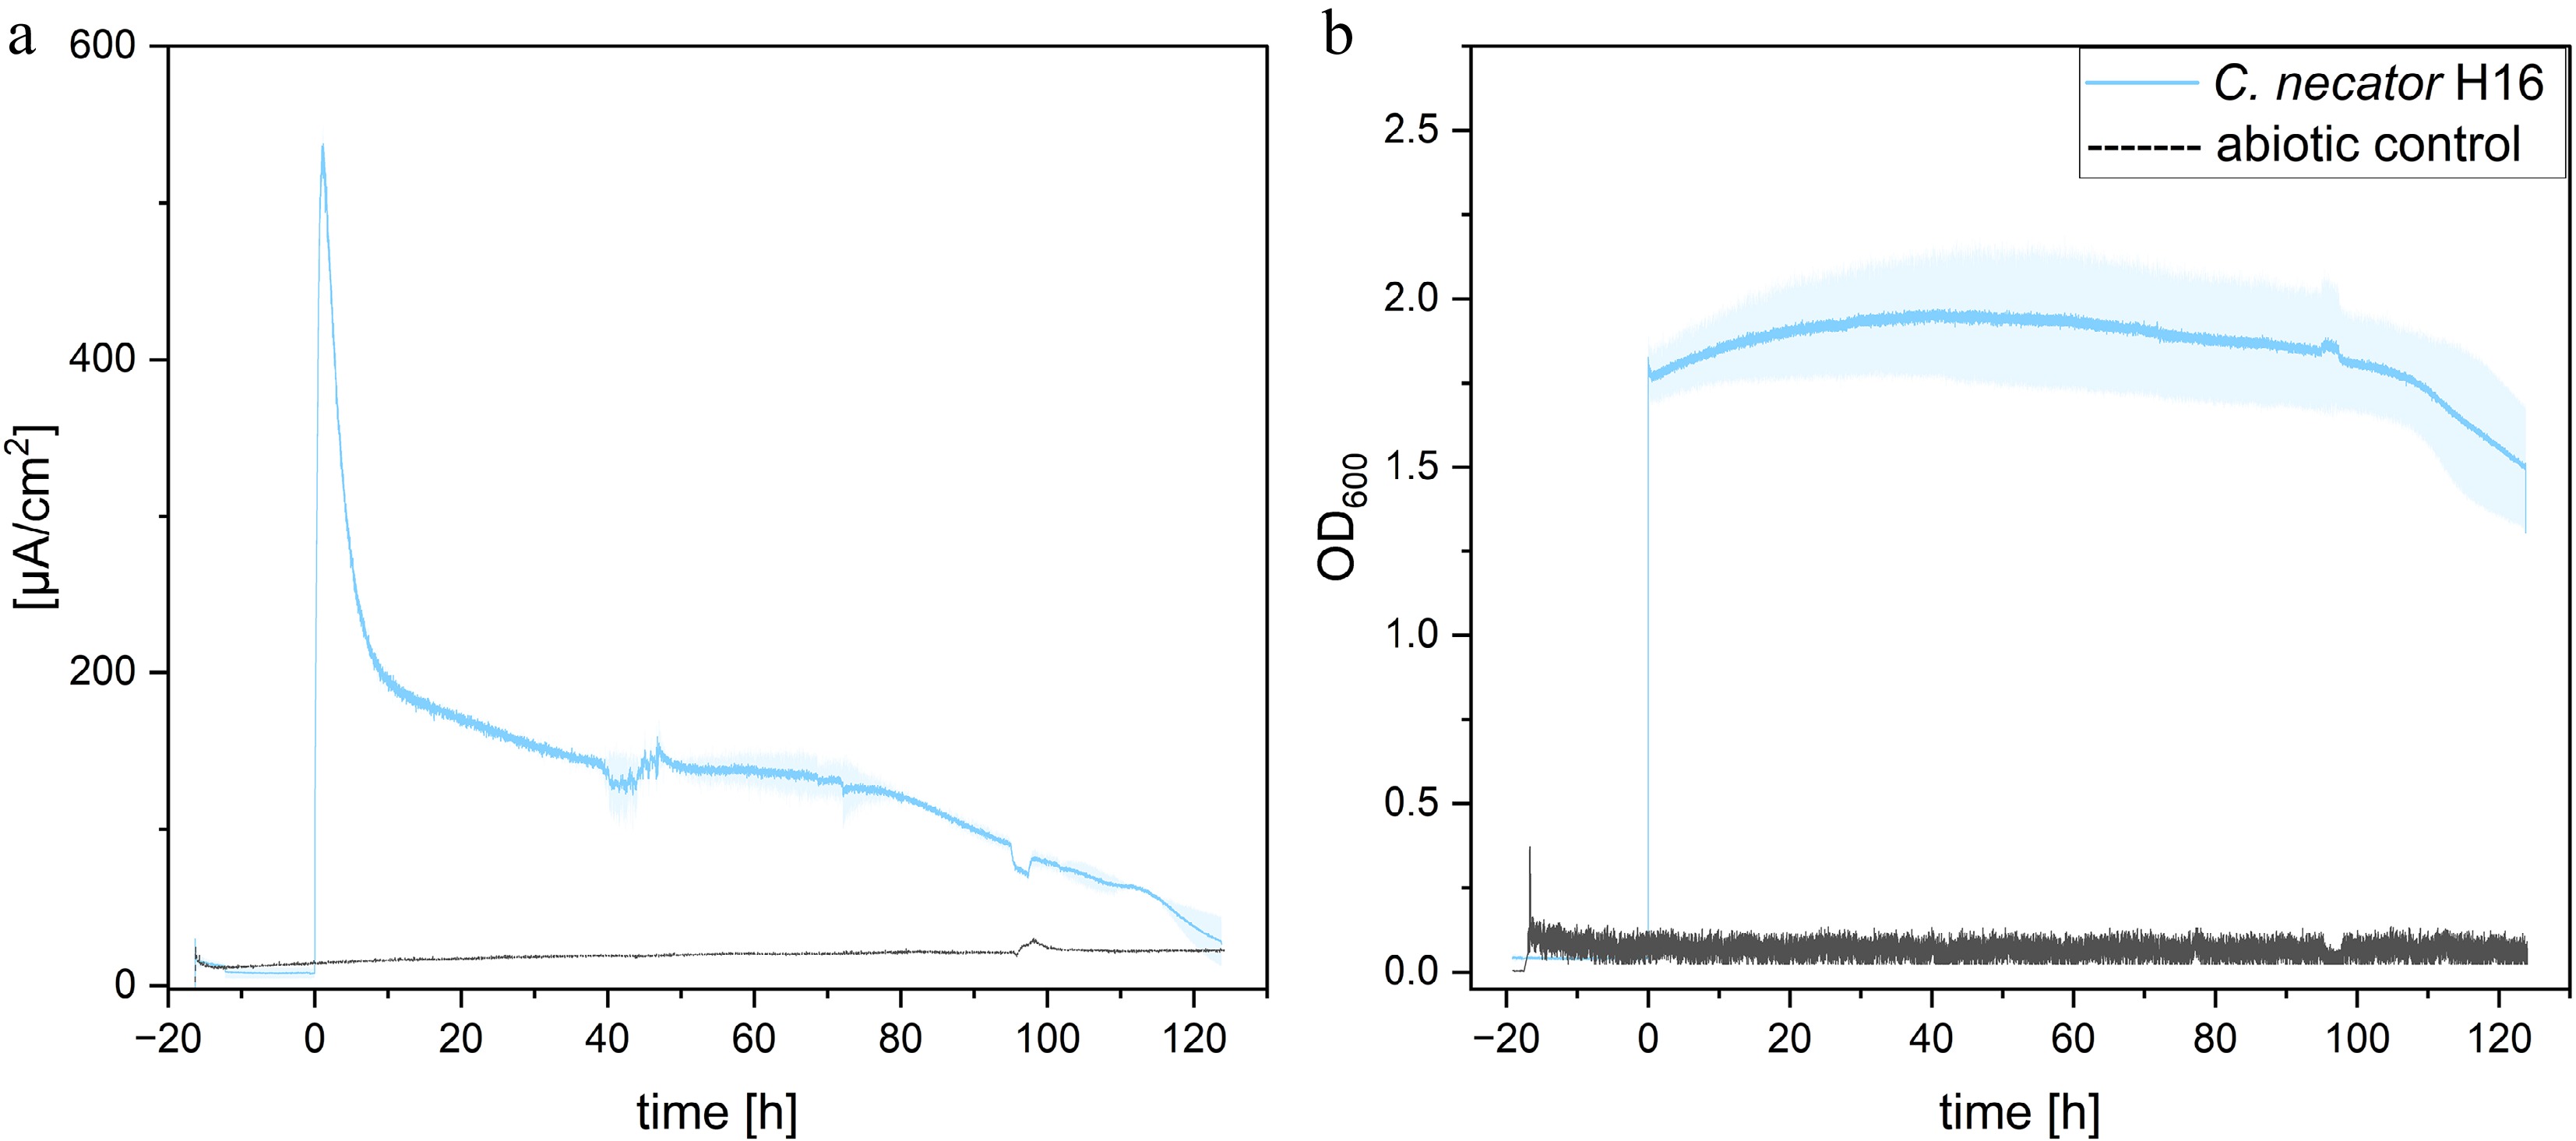
Figure 6.
Batch cultivation in the three-electrode Pioreactor®. C. necator H16 was cultivated in the electrified Pioreactor® in minimal medium with 5 mM FEC at 30 °C and 500 r/min for 9 d. A voltage of 500 mV was applied; the resulting current per electrode surface (a) lay around 150 µA/cm2 after recovery from a strong peak to 550 µA/cm2 at inoculation, till it reduced after 80 h of cultivation. The reactors were inoculated at an OD600 (b) of 1.75. An abiotic control is shown for the current density and optical density as a black graph (n = 1), the blue graphs show the inoculated experiments (n = 3).
-
Identifying a suitable small-scale system was the essential first step toward establishing an adaptation platform for electroactive bacteria, enabling semi-continuous or continuous operation, followed by the next requirement. The Pioreactor®[9] fulfils this role well, since integrated peristaltic pumps allow stable turbidostatic operation during bio-electrochemical cultivation with C. necator. A specialized cultivation system therefore called for an equally specialized adaptation approach. Using these reactor configurations, we performed adaptation under bio-electrochemical conditions and thereby established eALE.
With the herein introduced ePioreactor® and associated eALE, the size range separating liter-sized electro-bioreactors from e-cuvette-based screening formats could successfully be covered[3,4,6,31]. The developed mL-scale reactor shows a way to easily build a real possibility for an alternative to H-cells, applicable in different BES configurations with two or three electrodes, with the potential to be a standard for small-scale BES platforms. Especially, if the comparison to H-cells is drawn, a full process characterization is strongly suggested for further research to analyze specific parameters of both the one- and two-chamber setups, like kLa, mixing times, and ohmic resistance. With the benefits of the Pioreactor® as integrated photodiodes, heating, stirring, and liquid handling, as well as the possibility of parallelization by a Pioreactor® cluster, it is an ideal cost-effective reactor platform in electrobiotechnology. The possibility of a turbidostatic mode by using peristaltic pumps that come along with the reactor even makes eALE an option without extensive material and operating costs. By its size and the 3D-printable cast, the reactor is low in energy and material costs, as well as acquisition costs in the first place, which makes it a feasible option not only for professionals but also for student courses.
In the one-chamber setup, a turbidostatic cultivation with C. necator H16 ∆PHB was possible over a duration of nearly 10 d where medium supplemented with 350 mM sodium sulphate was fed into the reactor continuously (Fig. 3) resulting in a strain that showed under heterotrophic conditions, specifically in medium supplemented with 300 mM, enhanced growth compared to the parental strain (Fig. 4). Also, in the electro-autotrophic cultivation with the adapted strain vs. the parental strain supplemented with 300 mM of sodium sulphate, the adapted variant showed enhanced growth (Fig. 5). Therefore, the adaptation in an electrified Pioreactor® could be viewed as successful and stable, as after cryo-conservation and a seed train of three cultures, a difference in OD600 in both experiments (Figs. 4 and 5) could be observed. Nevertheless, sequencing and subsequent analysis would be inevitable for verifying genomic or transcriptomic changes due to adaptation, and are suggested for future research[32,33]. In the two-chamber setup, C. necator H16 was cultivated in minimal medium with fructose as a carbon and energy source with ferricyanide as a mediator for MET to the anode[14]. This system builds directly on the setup reported by Gemünde et al.[13]. Compared to the original system, where the cultivation was carried out in Dasgip reactors with 15 instead of 5 mM FEC, the cultivation time here was about 70 h shorter. But, like the original setup, there was a peak of current density at the inoculation time, which reduced over time. Overall, the current density in the ePioreactor® was more stable between 10 and 80 h after inoculation, lying around 150 µA/cm2, before it also decreased to around 0 between 80 and 120 h. The other parameters, such as the time course of the optical density, were comparable between the literature-reported data and our measured values. Therefore, it can be concluded that the developed electrified Pioreactor® is applicable for fast and efficient screening on a small scale. The system shown herein is a promising starting point for scale-up and an easily applicable platform for eALE. Besides the multiple advantages of the investigated reactor, there are still challenges that are yet to be solved, as in electrobiotechnological applications, often a pH control is needed, which is missing here.
In this work, we were able to show two electrified variations of the Pioreactor® and its use for fast adaptation under electro-autotrophic conditions. After a successful adaptation, a screening is usually the next step. Combining the eALE process in the electrified Pioreactor® with a platform enabling screening under electrobiological conditions, such as the previously reported e-cuvette system, would allow parallelized electrochemical screening[31]. To make sure the adapted strains are stable and to gain insights into genetic processes during electro-autotrophic cultivation, sequencing should be added to the spectrum of analytical tools after eALE experiments to dive deeper into mechanisms linked to electro-biochemistry. After eALE was shown in the one-chamber, two-electrode setup, an ideal possibility for future eALE in the herein introduced two-chamber/three-electrode setup would be the adaptation of C. necator to alternative redox mediators that might be non-toxic, for an even greener MET-based current production, without heavy pollutants that many redox mediators cause[34−36].
We have therefore introduced an eALE platform that can be used in at least two different configurations and has the potential to facilitate adaptation processes in electrobiotechnology involving different organisms, media, and electro-enzymatic applications. The developed reactor system is based on a commercial platform, bridging the gap between various custom-built setups by offering an easily applicable standard for electrobiotechnology. Furthermore, the reactor system could be used to investigate knowledge-based scaling up and identify suitable scale-up criteria for electro-bioreactors.
The authors gratefully acknowledge the financial support of Hector Stiftung.
-
During the preparation of this work, the author(s) used ChatGPT (free version/20.03.2026: 20.03.2026) for language refinement. The author(s) reviewed and edited all content produced with the assistance of this tool, verified its accuracy, and take full responsibility for the integrity and originality of the final manuscript. This work represents the author(s)' own intellectual contribution, and no AI tool is credited as an author.
-
The authors confirm their contributions to the paper as follows: study conception and design: van der Sande L, Maerz L; data collection: van der Sande L, Uhl T, Müller M; analysis and interpretation of results, draft manuscript preparation: van der Sande L, Holtmann D. All authors reviewed the results and approved the final version of the manuscript.
-
The data that support the findings of this study are available from the corresponding author upon reasonable request.
-
The authors declare that they have no conflict of interest.
-
accompanies this paper online at: https://doi.org/10.48130/els-0026-0012.
- Supplementary Fig. S1 Batch cultivation in the electrified Pioreactor® C. necator ΔPHB was cultivated in the electrified Pioreactor® under electro-autotrophic conditions in minimal medium at 30 °C and 500 rpm for 7 days.
- Supplementary Fig. S2 Calculated Na2SO4 concentration in mM during the continuous eALE process over time.
- Supplementary Table S1 Maximal specific growth rate of C. necator ΔPHB and the adePio variant during hours 6–20 of heterotrophic growth with different concentrations of sodium sulphate and statistical analysis via Welch-t-test (significant if p < 0.05).
- Copyright © 2026 by the author(s). Engineering in Life Sciences published by Maximum Academic Press on behalf of John Wiley & Sons Ltd. This is an open access article under the terms of the Creative Commons Attribution License, which permits use, distribution and reproduction in any medium, provided the original work is properly cited.
-
About this article
Cite this article
van der Sande L, Uhl T, Müller M, Maerz L, Holtmann D. 2026. An electrified small-scale bioreactor for different cultivation modes and adaptive laboratory evolution of Cupriavidus necator. Engineering in Life Sciences 26: e011 doi: 10.48130/els-0026-0012 
An electrified small-scale bioreactor for different cultivation modes and adaptive laboratory evolution of Cupriavidus necator
- Received: 09 April 2026
- Revised: 11 July 2026
- Accepted: 22 July 2026
- Published online: 14 September 2026
Abstract: Electrobiotechnology is increasingly recognized as a key platform technology for sustainable production processes, as it allows direct coupling of renewable electricity with biocatalysis, driving selective chemical transformations. One remaining challenge is the development of suitable reactors fulfilling both electrochemical and biocatalysis requirements. Conventional setups, often used as proof-of-concept, often represent negative examples regarding scalability and industrial relevance. Scalable, electrified bioreactors are needed for screening purposes and for large-scale bioproduction. This study presents a small-scale, electrified bioreactor (V = 20 mL) that can facilitate a variety of electrochemical conditions and bioprocess modes. Two reactor configurations based on the commercial Pioreactor® were established: a two-electrode one-chamber system for electro-autotrophic growth via in situ hydrogen production, and a three-electrode two-chamber system for anodic respiration via mediated electron transfer. Additionally, it was used for electrochemical adaptive laboratory evolution (eALE). Under turbidostatic electro-autotrophic conditions with gradually increasing sodium sulphate concentrations, an osmo-tolerant strain was obtained within 10 d. The adapted variant exhibited improved growth at 300 mM sodium sulphate compared to the parental strain, including reduced lag-phase and a higher final optical density. Cupriavidus necator was used as a model organism. Overall, the results suggest that the system establishes a viable connection between microtiter plates and established liter-scale bioreactor operations.