




-
The projected global population of 9 billion by 2050 is exerting unprecedented pressure on agricultural systems to satisfy rising food demand while ensuring environmental sustainability[1]. One key challenge is to enhance future food security without exacerbating adverse environmental impacts, particularly those arising from soil degradation induced by intensive agriculture[2,3]. In response to these daunting challenges, sustainable cropping systems centered on diversified rotations have emerged as promising alternatives to mitigate trade-offs between productivity and ecological balance[4,5]. Notably, the integration of legume species into low-input cropping systems is recognized as an effective win-win strategy, capable of reducing external nitrogen (N) inputs while sustaining or improving crop yields[6]. Although legume-based rotations are known to improve crop productivity and increase soil carbon (C) and N stocks[7,8], systematic evaluations of soil quality under such rotation systems are still scarce, particularly lacking in-depth investigations into soil quality variations across different soil layers.
Soil quality is a complex concept involving physical, chemical, and biological characteristics that collectively govern the soil's capacity to function within ecosystem boundaries, support biological productivity, and ensure environmental sustainability[2,9,10]. Soil organic carbon (SOC) is a fundamental indicator of soil quality, crucial for sustaining microbial activity and essential in nutrient cycling and climate regulation[11−13]. Research indicates that legume-based rotation increases both the proportion and C content of soil macroaggregates compared to continuous cereal cropping. This increase not only strengthens SOC sequestration and soil structural stability but also creates a favorable rhizosphere microenvironment for subsequent crops[7,14]. A meta-analysis indicated that incorporating leguminous crops into the cropping system can significantly increase SOC fractions[15]. However, SOC alone does not fully capture soil quality; N is equally important[3,8]. The distribution of soil C and N is highly dependent on depth and can be affected by crop residues, root biomass, and microbial activities[16,17]. Surface soils generally receive the majority of organic matter inputs and exhibit higher biological activity, whereas subsurface soils, despite having lower C and N contents, may store a substantial proportion of total stocks due to their greater volume[18,19]. Nevertheless, most existing studies have focused on the topsoil layer (0–20 cm), with insufficient attention paid to C, N, and other nutrient dynamics in deeper layers, which hinders a comprehensive and systematic evaluation of the soil quality evolution potential of legume-based rotation systems.
Soil extracellular enzymes are involved in nearly all soil biochemical reactions, and their activities act as a sensitive indicator of soil health and productivity, providing important insights into SOC sequestration and nutrient utilization[20,21]. As an important agricultural management practice, legume-based rotation can regulate the mineralization and release of exogenous C and N through diverse crop residues, thereby significantly shaping soil microbial community structure and extracellular enzyme activities[8,22,23]. Compared with cereal-cereal rotation, cereal-legume rotation can improve soil C and N availability and increase microbial biomass, thereby enhancing the activity of some key extracellular enzymes[1,8]. Meanwhile, a cereal-legume rotation can optimize microbial interactions and alleviate microbial resource limitations, further regulating enzyme-mediated nutrient transformation processes[24−26]. Therefore, clarifying the underlying mechanisms and ecological effects of soil extracellular enzyme stoichiometry under legume-based rotation is essential for enhancing soil quality and crop productivity.
A 14-year field experiment was conducted in the Huang-Huai-Hai Plain, involving three cropping systems: soybean–wheat rotation (SW), maize–wheat rotation (MW), and cotton–wheat rotation (CW). This study aimed to examine the impact of different rotation systems on SOC and TN stocks, extracellular enzyme activities, and soil quality at different soil depths. The following scientific hypotheses were proposed: (1) SW can more effectively enhance SOC and TN sequestration than non-legume rotations, and this positive effect gradually diminishes with increasing soil depth due to surface incorporation of soybean residues and relatively shallow root distribution; (2) SW can upregulate the activities of extracellular enzymes involved in C- and phosphorus (P)-acquiring processes but suppress N-acquiring enzymes due to improved soil N availability; (3) SW improves soil quality through coordinated alterations in soil nutrients and extracellular enzyme activities, with a significantly stronger response in the topsoil than in the subsoil.
-
In 2010, a long-term field experiment commenced at the National Field Research Station for Agricultural Ecosystems in Shangqiu, Henan Province, China (35°31′ N, 115°35′ E). This region has a warm temperate continental semi-humid monsoon climate, with an average annual precipitation of 708 mm and a mean annual temperature of 13.9 °C. The initial physicochemical properties of the 0–20 cm soil layer were reported by Wang et al.[27].
Three crop rotation systems were established in this study: SW, MW, and CW. Each treatment was replicated four times, with a plot area of 20 m2 (4 m × 5 m). Wheat was sown in late October and harvested between late May and early June of the next year. Soybean and maize were sown, and cotton seedlings were transplanted within 2 weeks after wheat harvest. Soybean and maize were cultivated via direct seeding, whereas cotton was grown using the seedling transplanting method. All three crops were harvested in October of the same year. For soybean, cotton, and maize, only the underground residues were processed and mixed into the soil after removing the aboveground plant parts. Wheat straw was chopped into segments of about 10 cm in length and returned to the field. The application rates for wheat were 225 kg N ha−1, 90 kg P2O5 ha−1, and 105 kg K2O ha−1; for soybean, the rates were 90 kg N ha−1, 120 kg P2O5 ha−1, and 60 kg K2O ha−1; for maize and cotton, the rates were identical, with 180 kg N ha−1, 120 kg P2O5 ha−1, and 60 kg K2O ha−1. All other field management practices for pest and disease control adhered to local conventional agronomic practices.
Soil sample collection and processing
-
In May 2024, soil samples were obtained from each experimental plot at two depth intervals: 0–20 cm (topsoil) and 20–40 cm (subsoil). Subsequently, the soil samples collected from each treatment plot were thoroughly mixed to ensure compositional uniformity. All soil samples were passed through a 2-mm sieve to remove large impurities such as root debris and stones. Each sample was then split into two subsamples: one stored at 4 °C for immediate analysis of soil microbial properties and extracellular enzyme activities; the other air-dried at room temperature for determination of soil physicochemical properties.
Soil physicochemical characteristics
-
The potassium dichromate volumetric method was employed for the quantification of SOC, and soil TN was determined following the modified Kjeldahl procedure[28]. The determination of soil dissolved organic C (DOC) followed the methodology outlined by Jones & Willett[29]. The chloroform fumigation technique was employed for the determination of soil microbial biomass C (MBC) and N (MBN)[30]. Ammonium N (NH4+-N) and nitrate N (NO3−-N) contents were determined using a continuous flow analyzer[19]. Soil available P (AP) was quantified through HCl–H2SO4 extraction and subsequent molybdenum blue colorimetry[31]. Soil pH was measured using a pH meter in a 1:2.5 (w/v) soil-to-water suspension. Soil aggregates with particle size larger than 0.25 mm (R0.25) were isolated via the wet-sieving procedure[3]. Soil bulk density (BD) was calculated by dividing the mass of oven-dried soil by its respective volume. For each soil layer, the stocks of SOC and TN were calculated by multiplying their respective concentrations by the corresponding BD.
Soil extracellular enzymes
-
The activities of β-glucosidase (BG), cellobiosidase (CBH), β-N-acetyl-glucosaminidase (NAG), L-leucine aminopeptidase (LAP), alkaline phosphatase (AKP), and phenol oxidase (PHO) were measured as described by Hu & Liu[32,33]. Enzyme activities were assessed through microplate-based fluorometric and photometric methods. Hydrolytic enzymes (BG, CBH, NAG, LAP, and AKP) were assayed with 4-methylumbelliferone (MUB)- and 7-amino-4-methylcoumarin (AMC)-linked fluorogenic substrates, while PHO was determined using L-DOPA as the substrate. All samples were incubated in the dark at 25 °C for 3 h for hydrolase reactions and 5 h for oxidase reactions. Hydrolase activity was measured using a microplate reader with fluorescence detection at 360 nm excitation and 460 nm emission wavelengths. Oxidase activity was evaluated by measuring absorbance at 450 nm.
The vector length and vector angle of soil extracellular enzyme stoichiometry were calculated as follows[11]:
$ \begin{split}\rm Vector\;length =\;&\rm SQRT \Bigg[\left(\dfrac{BG + CBH}{BG+CBH+AKP}\right)^2+\\&\rm\left(\dfrac{BG+CBH}{BG+CBH+NAG+LAP}\right)^2\Bigg] \end{split}$ (1) $ \begin{split} \rm{V}ector\; angle=\; & \rm{D}EGREES\Bigg[ATAN2\Bigg(\dfrac{BG+CBH}{BG+CBH+AKP}+ \\ &\rm{\dfrac{BG+CBH}{BG+CBH+NAG+LAP}}\Bigg)\Bigg]\ , \end{split} $ (2) where, vector length represents the relative microbial demand for C, and vector angle reflects the relative demand for P vs N. A vector angle greater than 45° indicates a relatively higher demand for P compared with N, whereas an angle less than 45° indicates a relatively higher demand for N.
Soil quality assessment
-
To assess the comprehensive effects of long-term rotation systems, this study adopted the soil quality index-area (SQI–area) approach to calculate SQI[11,34]. The basic dataset selected in the study included 10 soil indicators (physical indicators: R0.25; chemical indicators: SOC stock, TN stock, DOC, NO3−-N, NH4+-N, AP, pH; biological indicators: MBC, MBN). In the SQI calculation process, all physical, chemical, and biological indicators were normalized to a 0–1 scale. Indicators were classified into two groups based on their contribution to soil quality. The 'higher is better' scoring rule (Eq. [3]) was applied to SOC stock, TN stock, DOC, NO3−-N, NH4+-N, AP, R0.25, MBC, and MBN, as higher values of these indicators reflect greater nutrient availability and microbial activity. The 'lower is better' rule (Eq. [4]) was applied to pH because the tested soil is alkaline (pH > 8.0), and lower pH values within range favor nutrient availability:
$ {\text{SI}}_{n}=\dfrac{X}{{X}_{\max }} $ (3) $ {\text{SI}}_{n}=\dfrac{{X}_{\min }}{X} $ (4) $ \text{SQI = 0.5×}\sum\nolimits_{n}^{i}\text{SI}_{n}^{2}\times \sin \left(\frac{\text{2π}}{i}\right), $ (5) where, SIn is the linear score of indicator n, 0–1; X, Xmax, and Xmin are the measured, max, and min values of indicator n, respectively. i represents the total number of parameters included in the SQI.
Statistical analysis
-
To account for the non-independence of topsoil and subsoil samples from the same plots, linear mixed-effects models were fitted using the 'lme4' package in R (v4.3.2), with rotation system, soil depth, and their interaction as fixed effects, and block and plot nested within block as random effects. Fixed-effect significance was determined using Satterthwaite's method (via 'lmerTest'), and pairwise comparisons were conducted using 'emmeans' with Tukey's HSD adjustment (p < 0.05). Pearson correlation analysis between SQI and extracellular enzyme activities was performed using the 'corrplot' package in R.
-
Compared with MW and CW, SW significantly increased SOC stock by 12.4%–17.2%, TN stock by 13.4%–15.9%, DOC content by 25.6%–42.4%, NO3−-N content by 11.6%–47.2%, AP content by 14.9%–24.9%, MBC content by 13.4%–16.4%, and MBN content by 17.1%–21.9% in the topsoil layer, and significantly decreased soil pH (Fig. 1). Compared with MW, CW significantly elevated topsoil DOC content by 13.4% and NO3−-N content by 31.9%, and caused a significant reduction in soil pH. In the subsoil layer, relative to MW and CW, SW significantly increased AP content by 16.8%–26.2% and MBN content by 21.9%–35.1%, but markedly decreased soil pH and the microbial biomass carbon-to-nitrogen ratio (MBC:N) (Fig. 1). Compared with MW, SW significantly enhanced subsoil TN stock by 6.2% and DOC content by 9.1%, whereas no significant differences were detected between SW and CW. Notably, BD showed no significant differences among all treatments in either the topsoil or subsoil layer. Across the entire soil layer (0–40 cm), with the exception of NH4+-N, nutrient contents and microbial biomass were typically higher in the topsoil than in the subsoil.
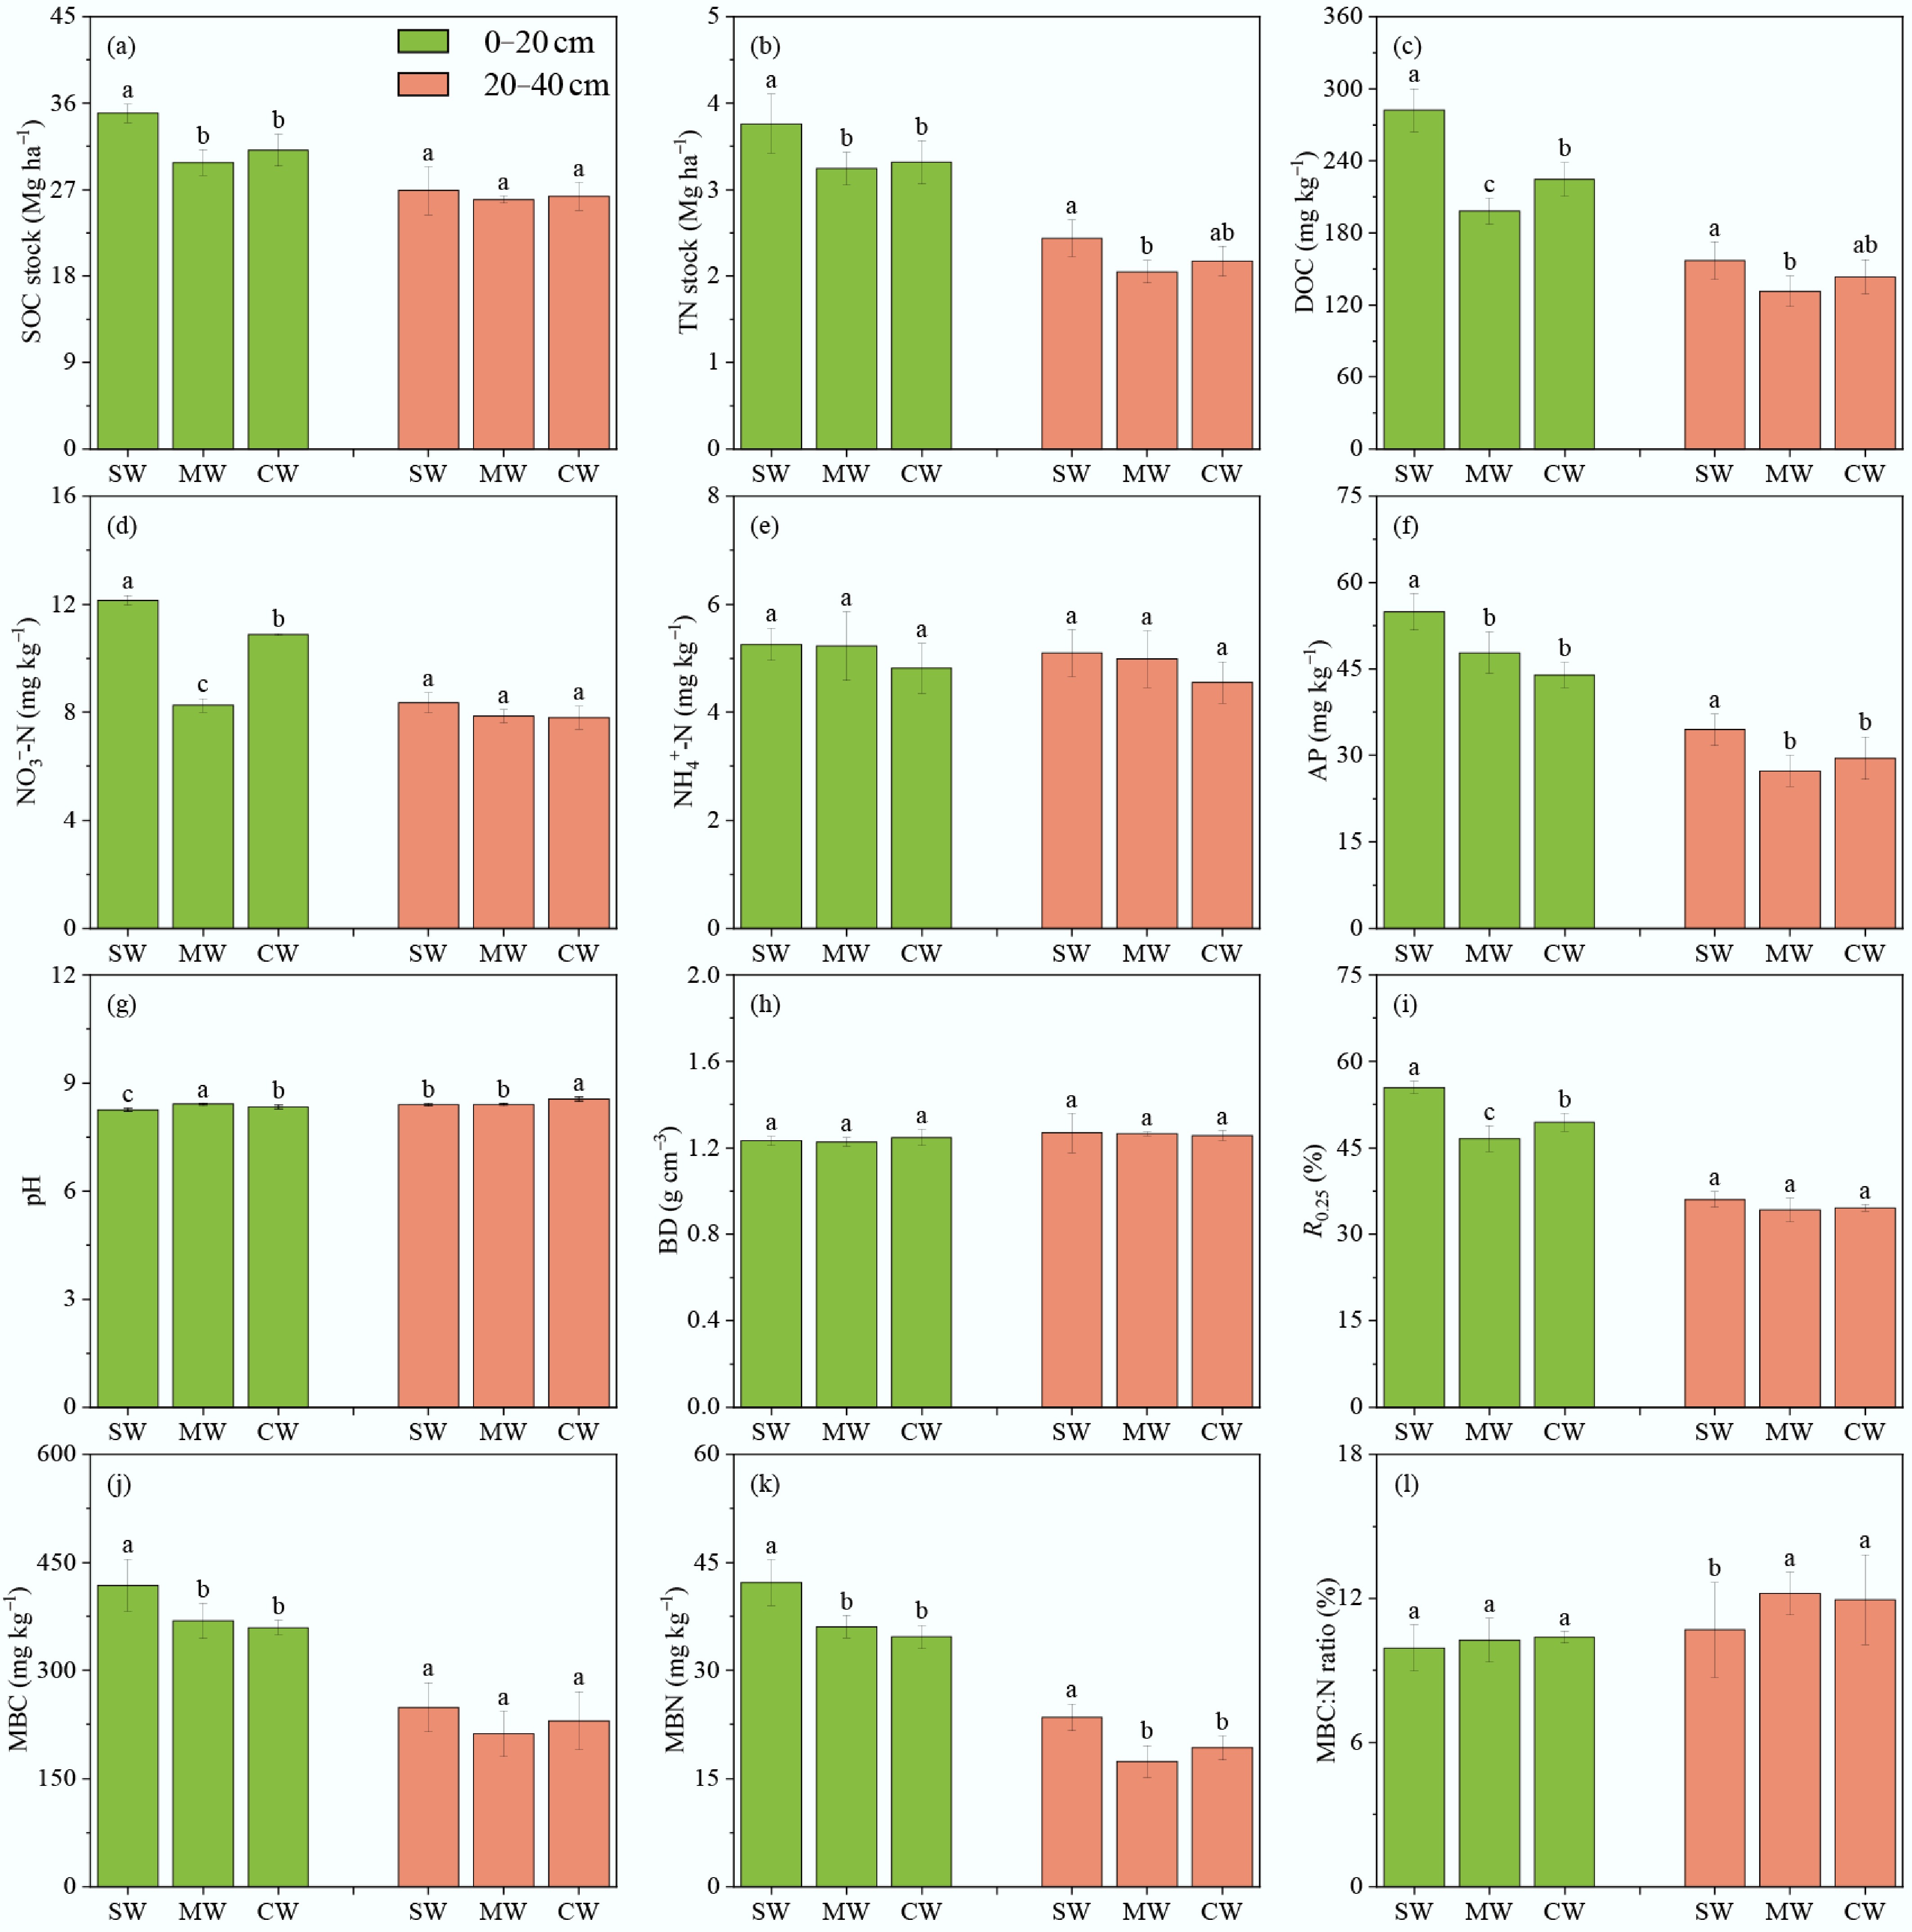
Figure 1.
Soil abiotic and biotic properties in different crop rotation patterns. Values are means ± standard error (n = 4). Significant differences among treatments at p < 0.05 are indicated by lowercase letters. SW, soybean–wheat rotation; MW, maize–wheat rotation; CW, cotton–wheat rotation. SOC, soil organic carbon; TN, total nitrogen; DOC, dissolved organic carbon; NO3−-N, nitrate nitrogen; NH4+-N, ammonium nitrogen; AP, available phosphorus; BD, bulk density; R0.25, > 0.25 mm aggregates; MBC, microbial biomass carbon; MBN, microbial biomass nitrogen; MBC:N, microbial biomass carbon-to-nitrogen ratio.
Soil extracellular enzyme activities and stoichiometry
-
In the topsoil layer, compared with MW and CW, SW significantly increased the activity of BG by 27.6%–38.1%, CBH by 37.7%–47.7%, and AKP by 43.7%–45.7% (Fig. 2). Relative to MW, SW markedly improved NAG activity by 12.9%, whereas no significant difference was observed between SW and CW. Compared with CW, SW markedly elevated PHO activity by 25.2%, while no significant difference was observed between SW and MW. In the subsoil layer, compared with MW and CW, SW significantly increased CBH activity by 25.2%–28.8%, AKP activity by 15.9%–22.3%, and PHO activity by 31.3%–42.8% (Fig. 2). Compared with MW, SW significantly improved NAG activity by 23.7%. Notably, none of the tested soil enzyme activities differed significantly between MW and CW in the subsoil layer. Throughout the 0–40 cm soil layer, extracellular enzyme activities were typically greater in the topsoil compared with the subsoil.
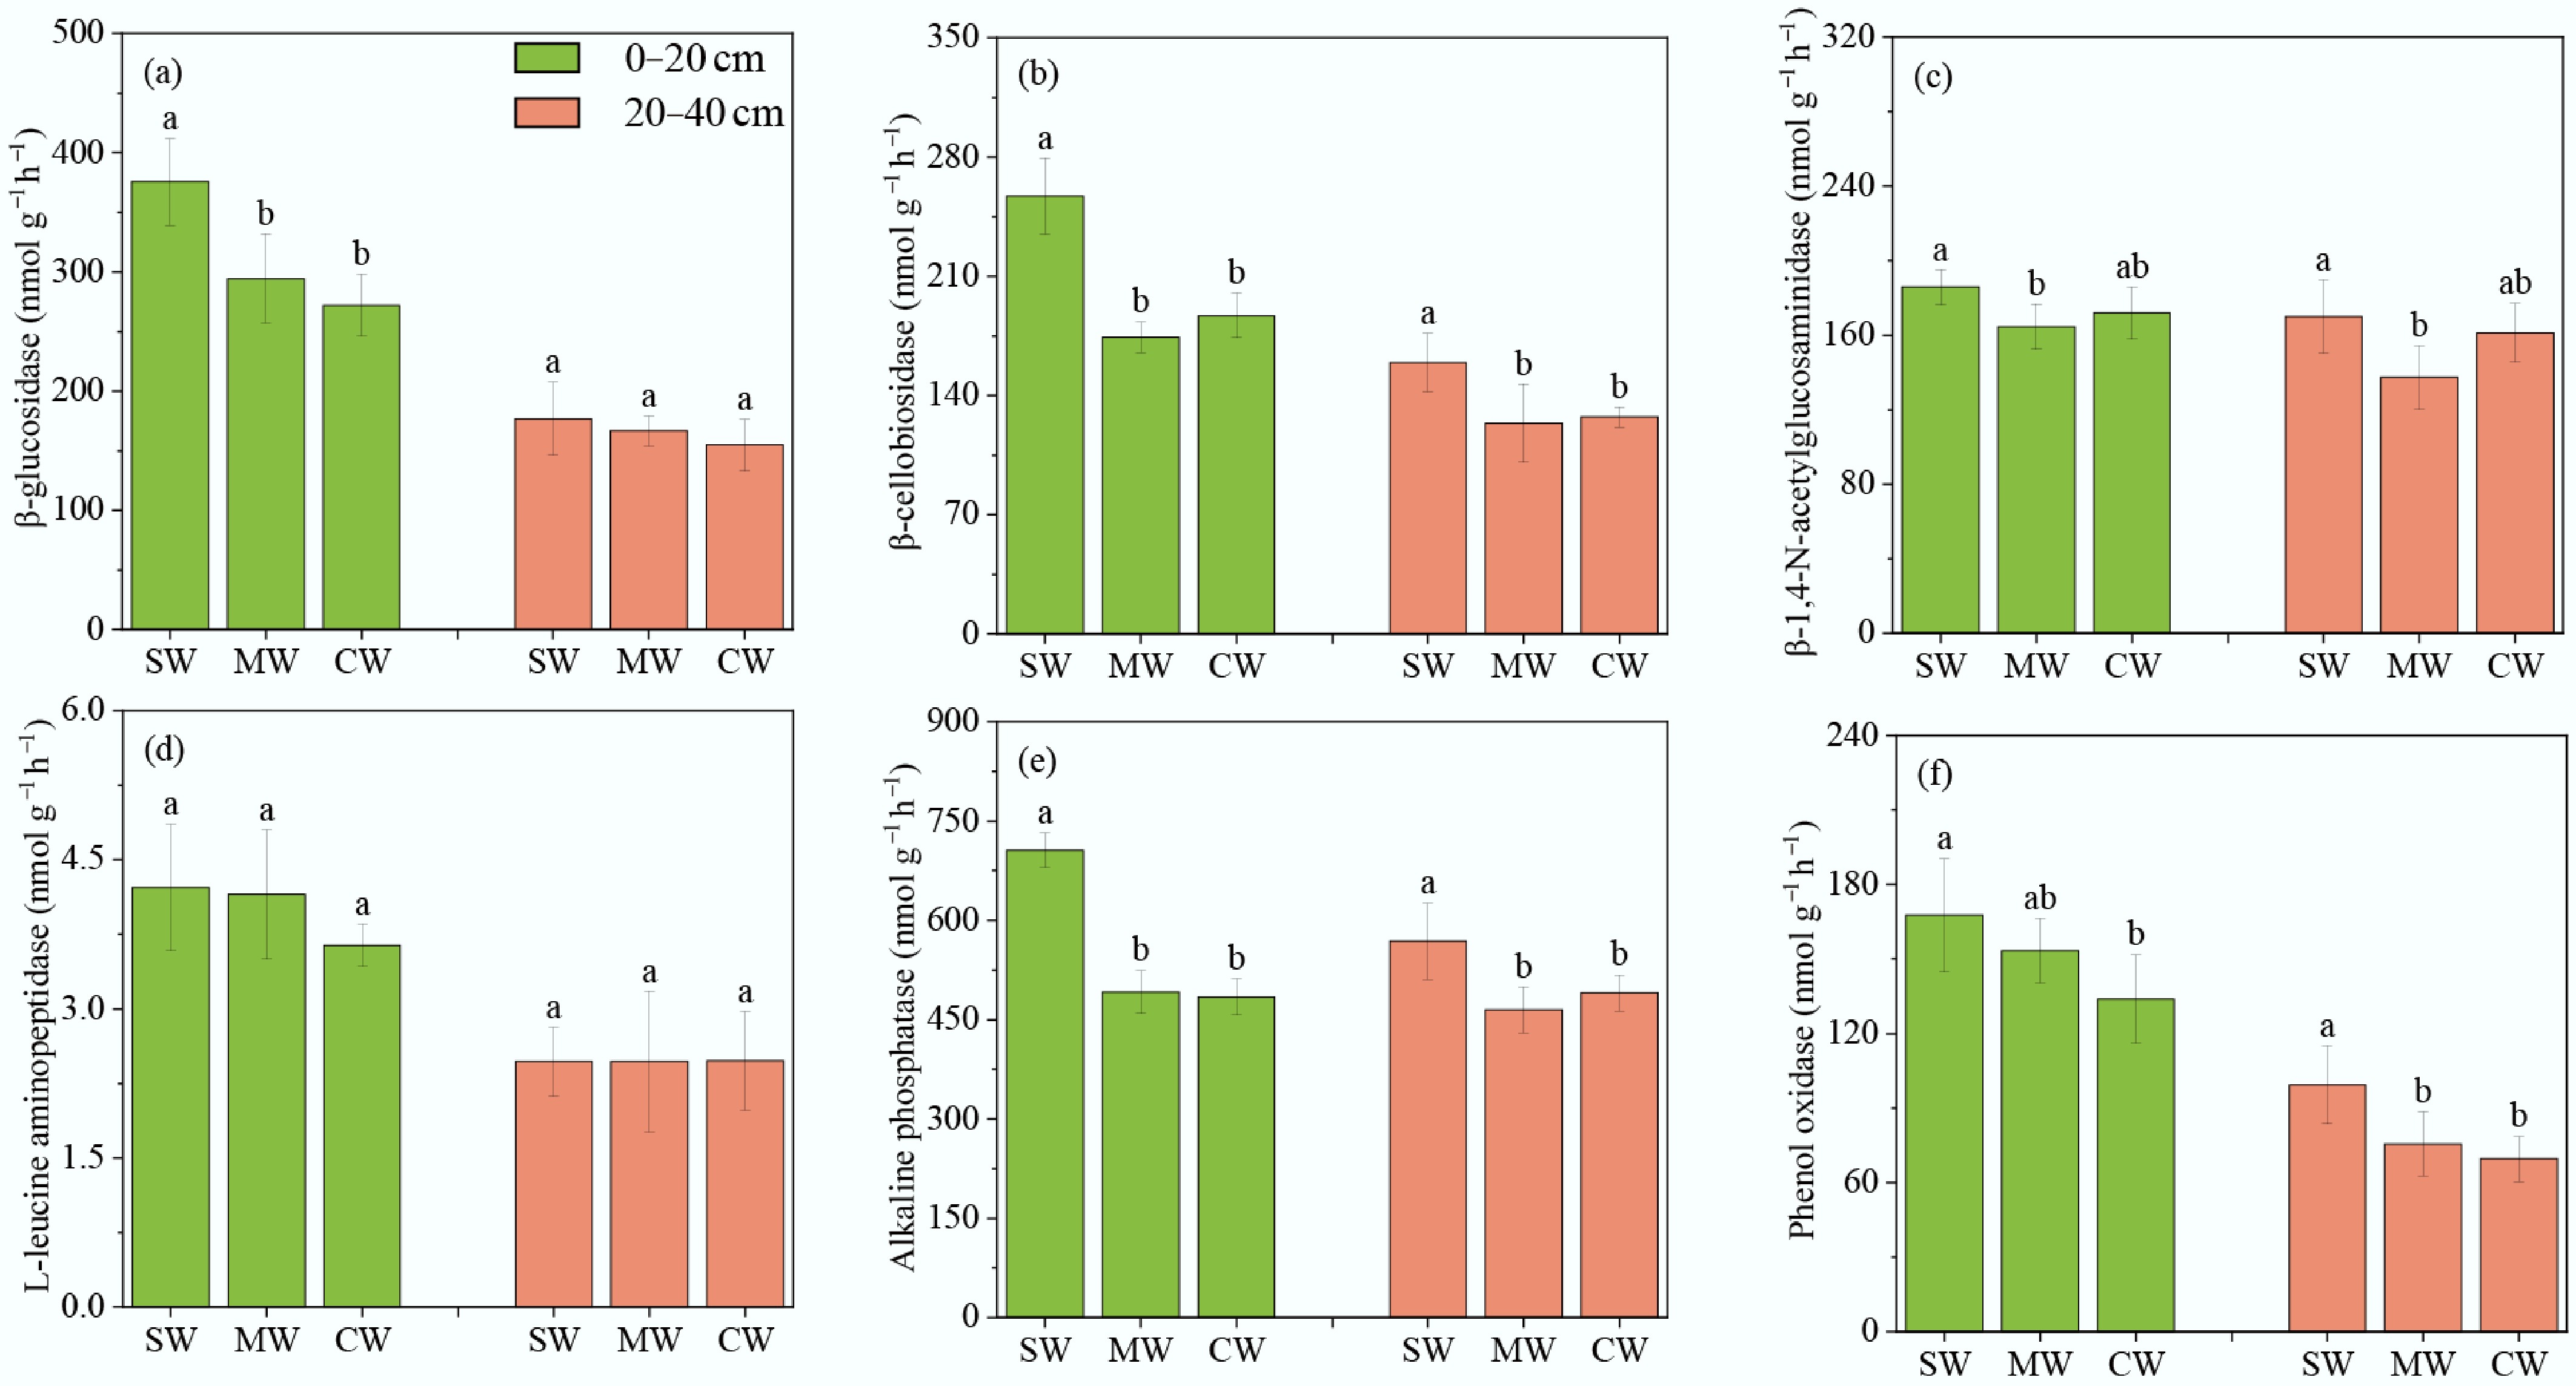
Figure 2.
Soil extracellular enzyme activities under different rotation patterns. Values are means ± standard error (n = 4). Significant differences among treatments at p < 0.05 are indicated by lowercase letters. SW, soybean–wheat rotation; MW, maize–wheat rotation; CW, cotton–wheat rotation.
The response patterns of soil enzyme stoichiometry ratios in the topsoil exhibited significant divergence among different rotation patterns (Fig. 3a). Under all rotation patterns, the vector angles of soil enzyme stoichiometry surpassed 45°, indicating a relatively high microbial investment in P acquisition within the study area. Compared with non-leguminous crop rotation systems, the vector angles of SW increased significantly by 3.6%–4.2%, suggesting higher relative microbial investment in P acquisition (Fig. 3c). In addition, vector lengths, which reflect the relative microbial investment in C acquisition, did not differ significantly across the rotation systems (Fig. 3b), indicating that crop rotation had no significant effect on microbial C investment. A significant negative relationship was identified between vector length and vector angle (Fig. 3d), suggesting a trade-off in microbial resource allocation between C and P/N acquisition.
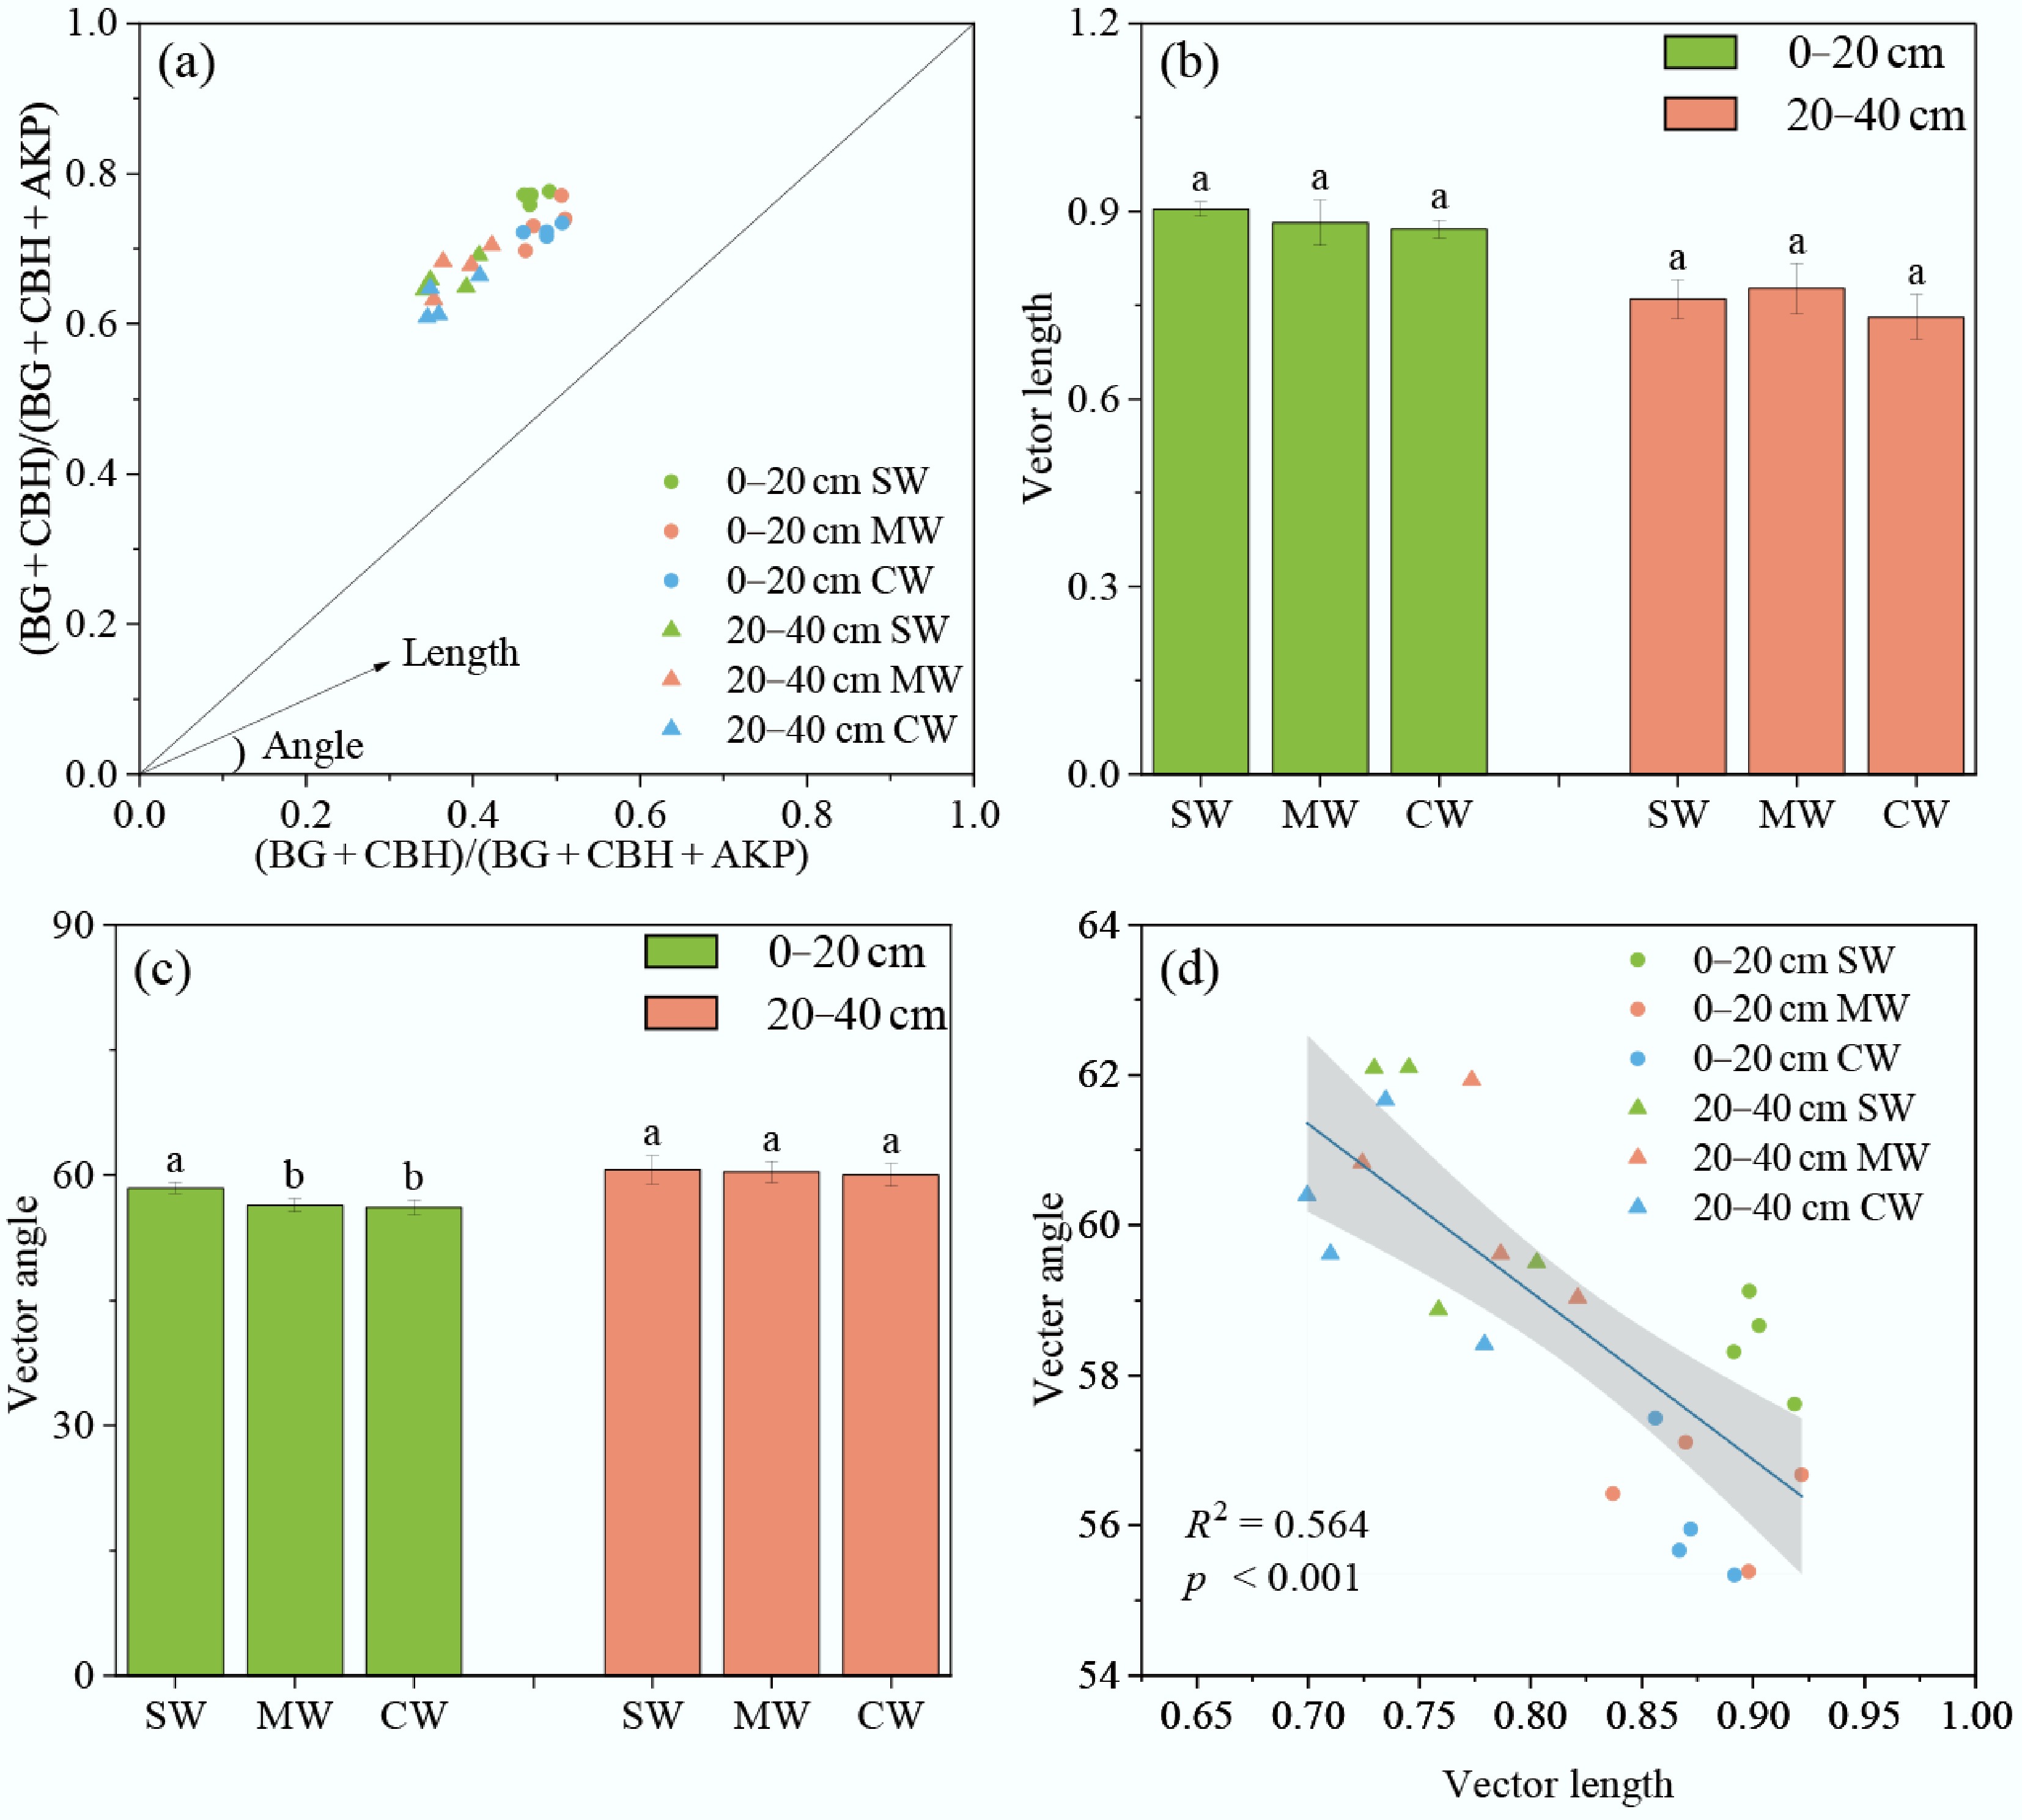
Figure 3.
Enzyme stoichiometry under different rotation patterns. (a) Vector length denotes microbial carbon limitation. (b) Vector angle indicates microbial nitrogen limitation (< 45°) or phosphorus limitation (> 45°). (c) Regression analysis of the relationships between microbial carbon limitation (vector length) and microbial nitrogen or phosphorus limitation (vector angle). (d) Values are the means ± standard error (n = 4). Significant differences among treatments at p < 0.05 are indicated by lowercase letters. SW, soybean–wheat rotation; MW, maize–wheat rotation; CW, cotton–wheat rotation.
Soil quality index
-
SQI is a crucial indicator for assessing the sustainability of soil ecosystems. Linear mixed-effects models showed that the rotation system significantly affected SQI, whereas soil depth and its interaction had no significant effects (Supplementary Table S1). Compared with MW and CW, SW significantly increased SQI by 30.0%–36.7% in the topsoil and by 18.5%–24.3% in the subsoil (Fig. 4). However, SQI did not differ significantly between MW and CW. SQI showed a significantly positive relationship with soil vector angle, while no significant correlation was detected between SQI and vector length (Fig. 5). Correlation analysis demonstrated that in the topsoil, SQI was markedly correlated with BG, CBH, NAG, AKP, and vector angle (Fig. 6a). In the subsoil, SQI was significantly correlated with CBH, AKP, and PHO (Fig. 6b).
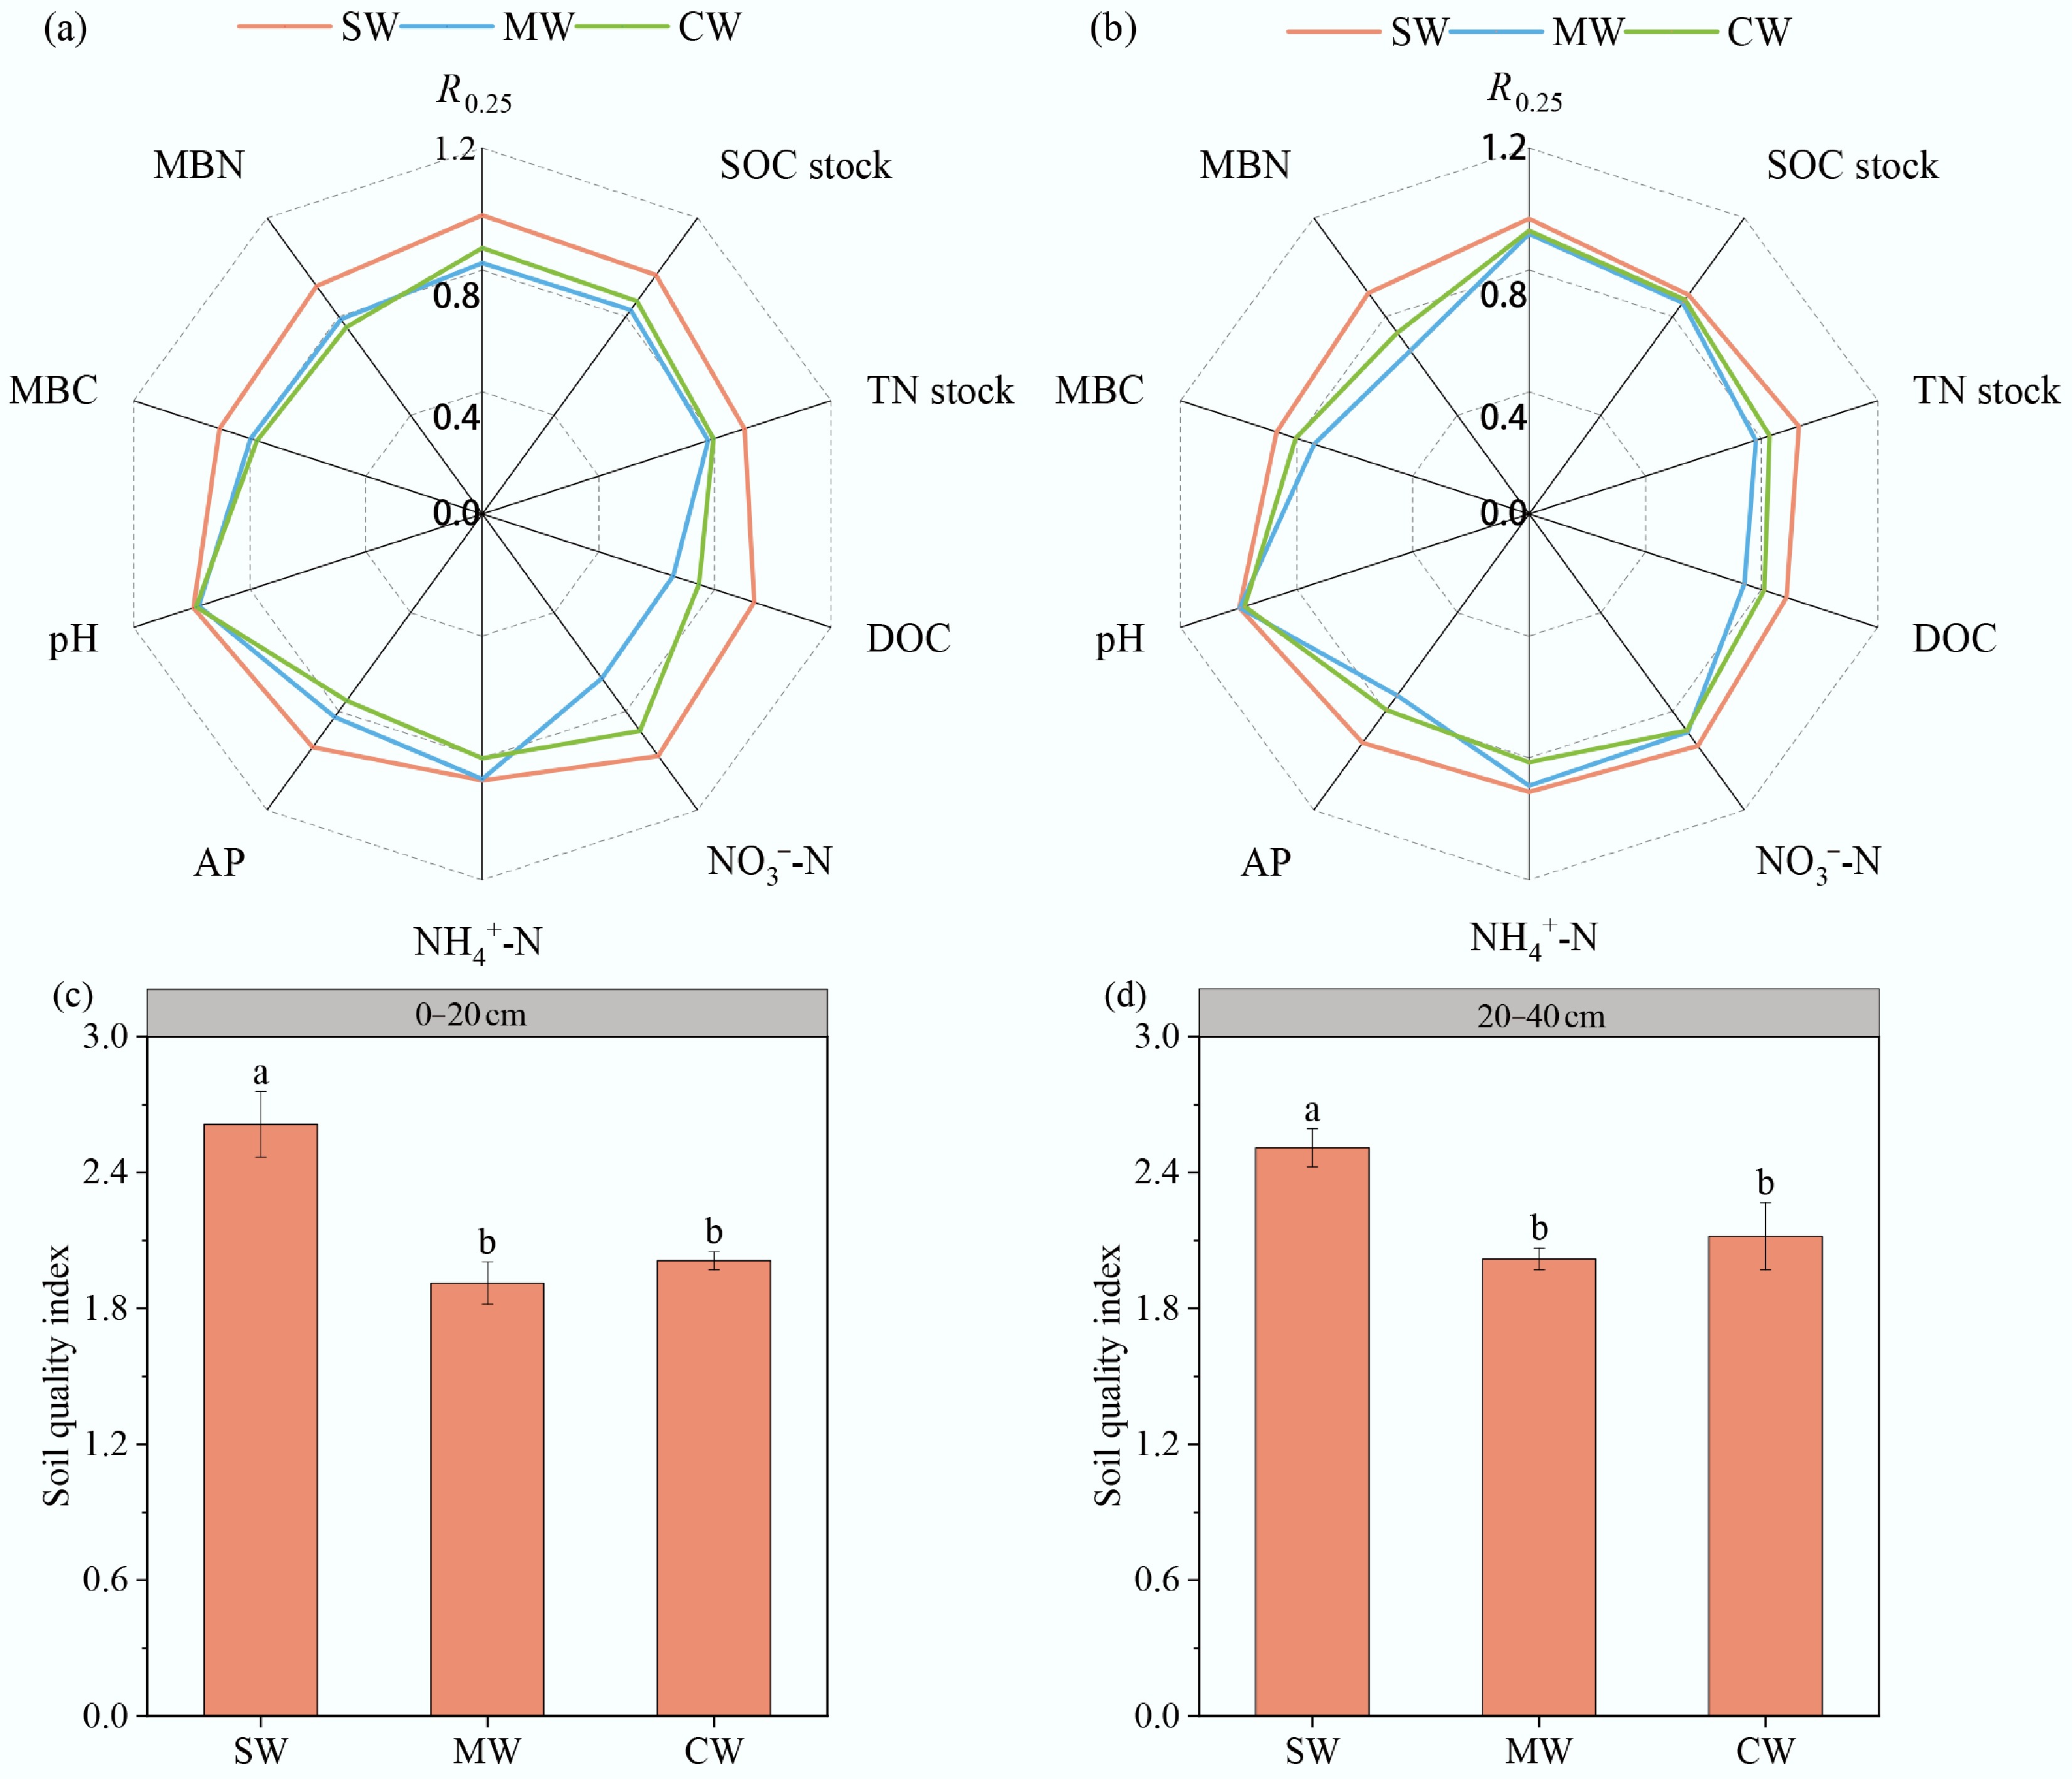
Figure 4.
Standardized comparison of soil abiotic and biotic properties in the (a) topsoil (0–20 cm), and (b) subsoil (20–40 cm); soil quality index under different rotation systems in the (c) topsoil and (d) subsoil. Values are the means ± standard error (n = 4). Significant differences among treatments at p < 0.05 are indicated by lowercase letters. SW, soybean–wheat rotation; MW, maize–wheat rotation; CW, cotton–wheat rotation. SOC, soil organic carbon; TN, total nitrogen; DOC, dissolved organic carbon; NO3−-N, nitrate nitrogen; NH4+-N, Ammonium nitrogen; AP, available phosphorus; R0.25, > 0.25 mm aggregates; MBC, microbial biomass carbon; MBN, microbial biomass nitrogen.
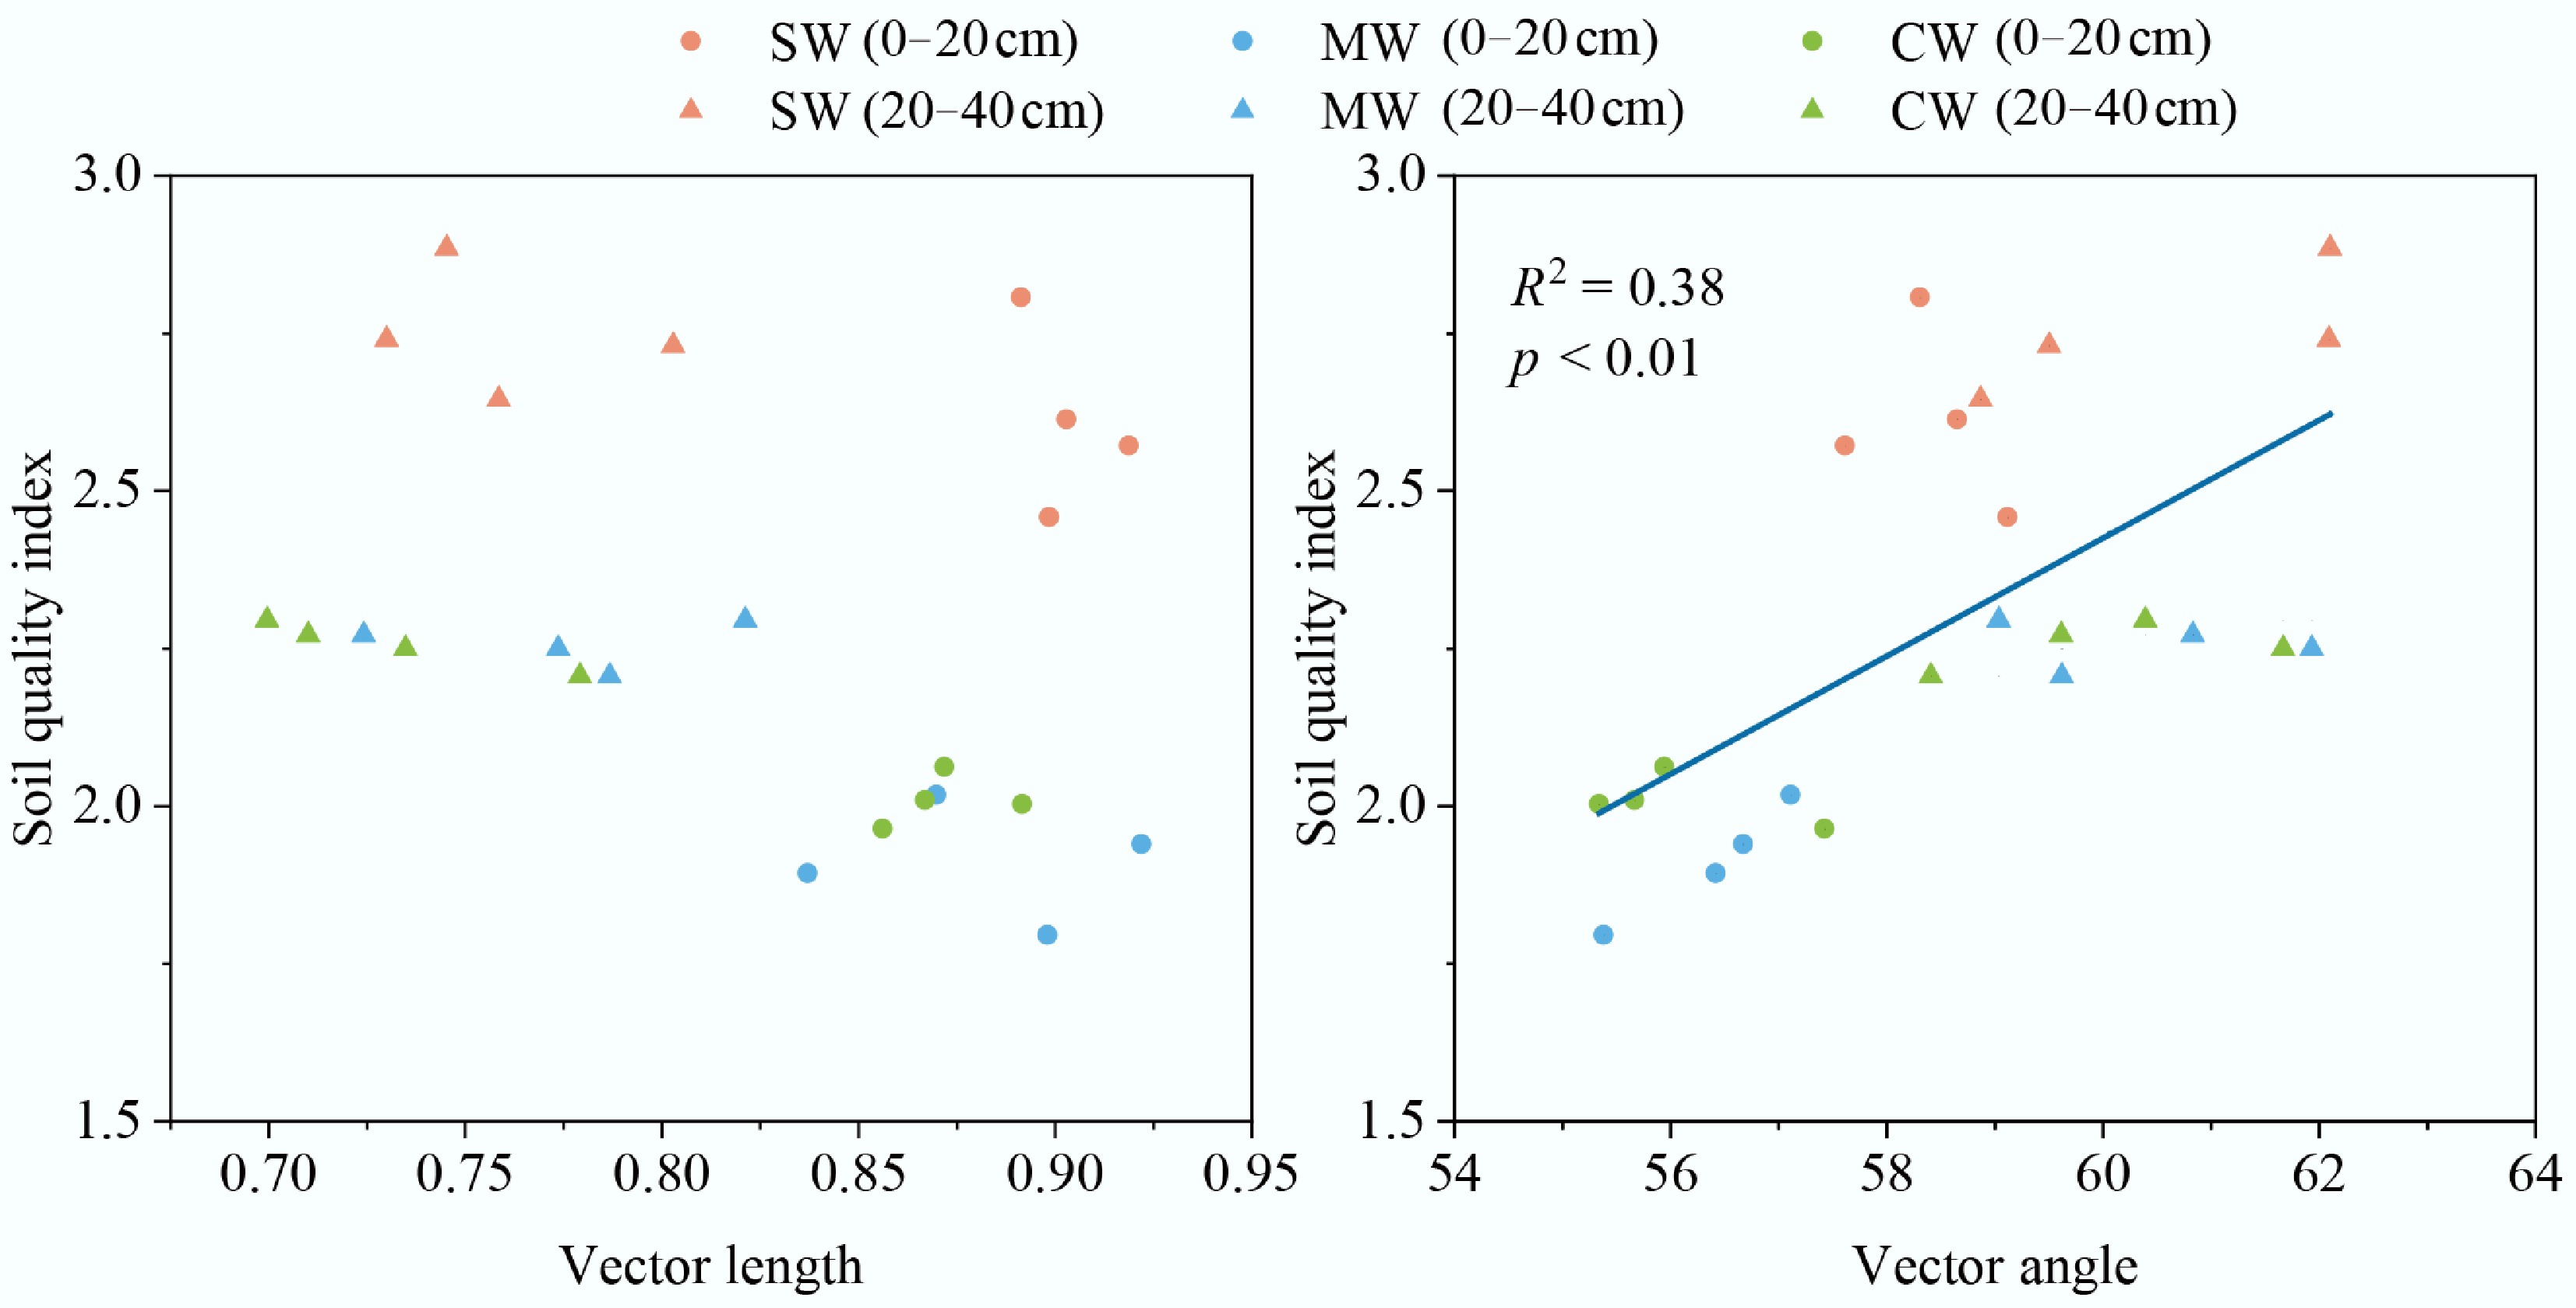
Figure 5.
Linear relationships between soil quality index and vector length (microbial carbon limitation) and vector angle (microbial nitrogen or phosphorus limitation). SW, soybean–wheat rotation; MW, maize–wheat rotation; CW, cotton–wheat rotation.
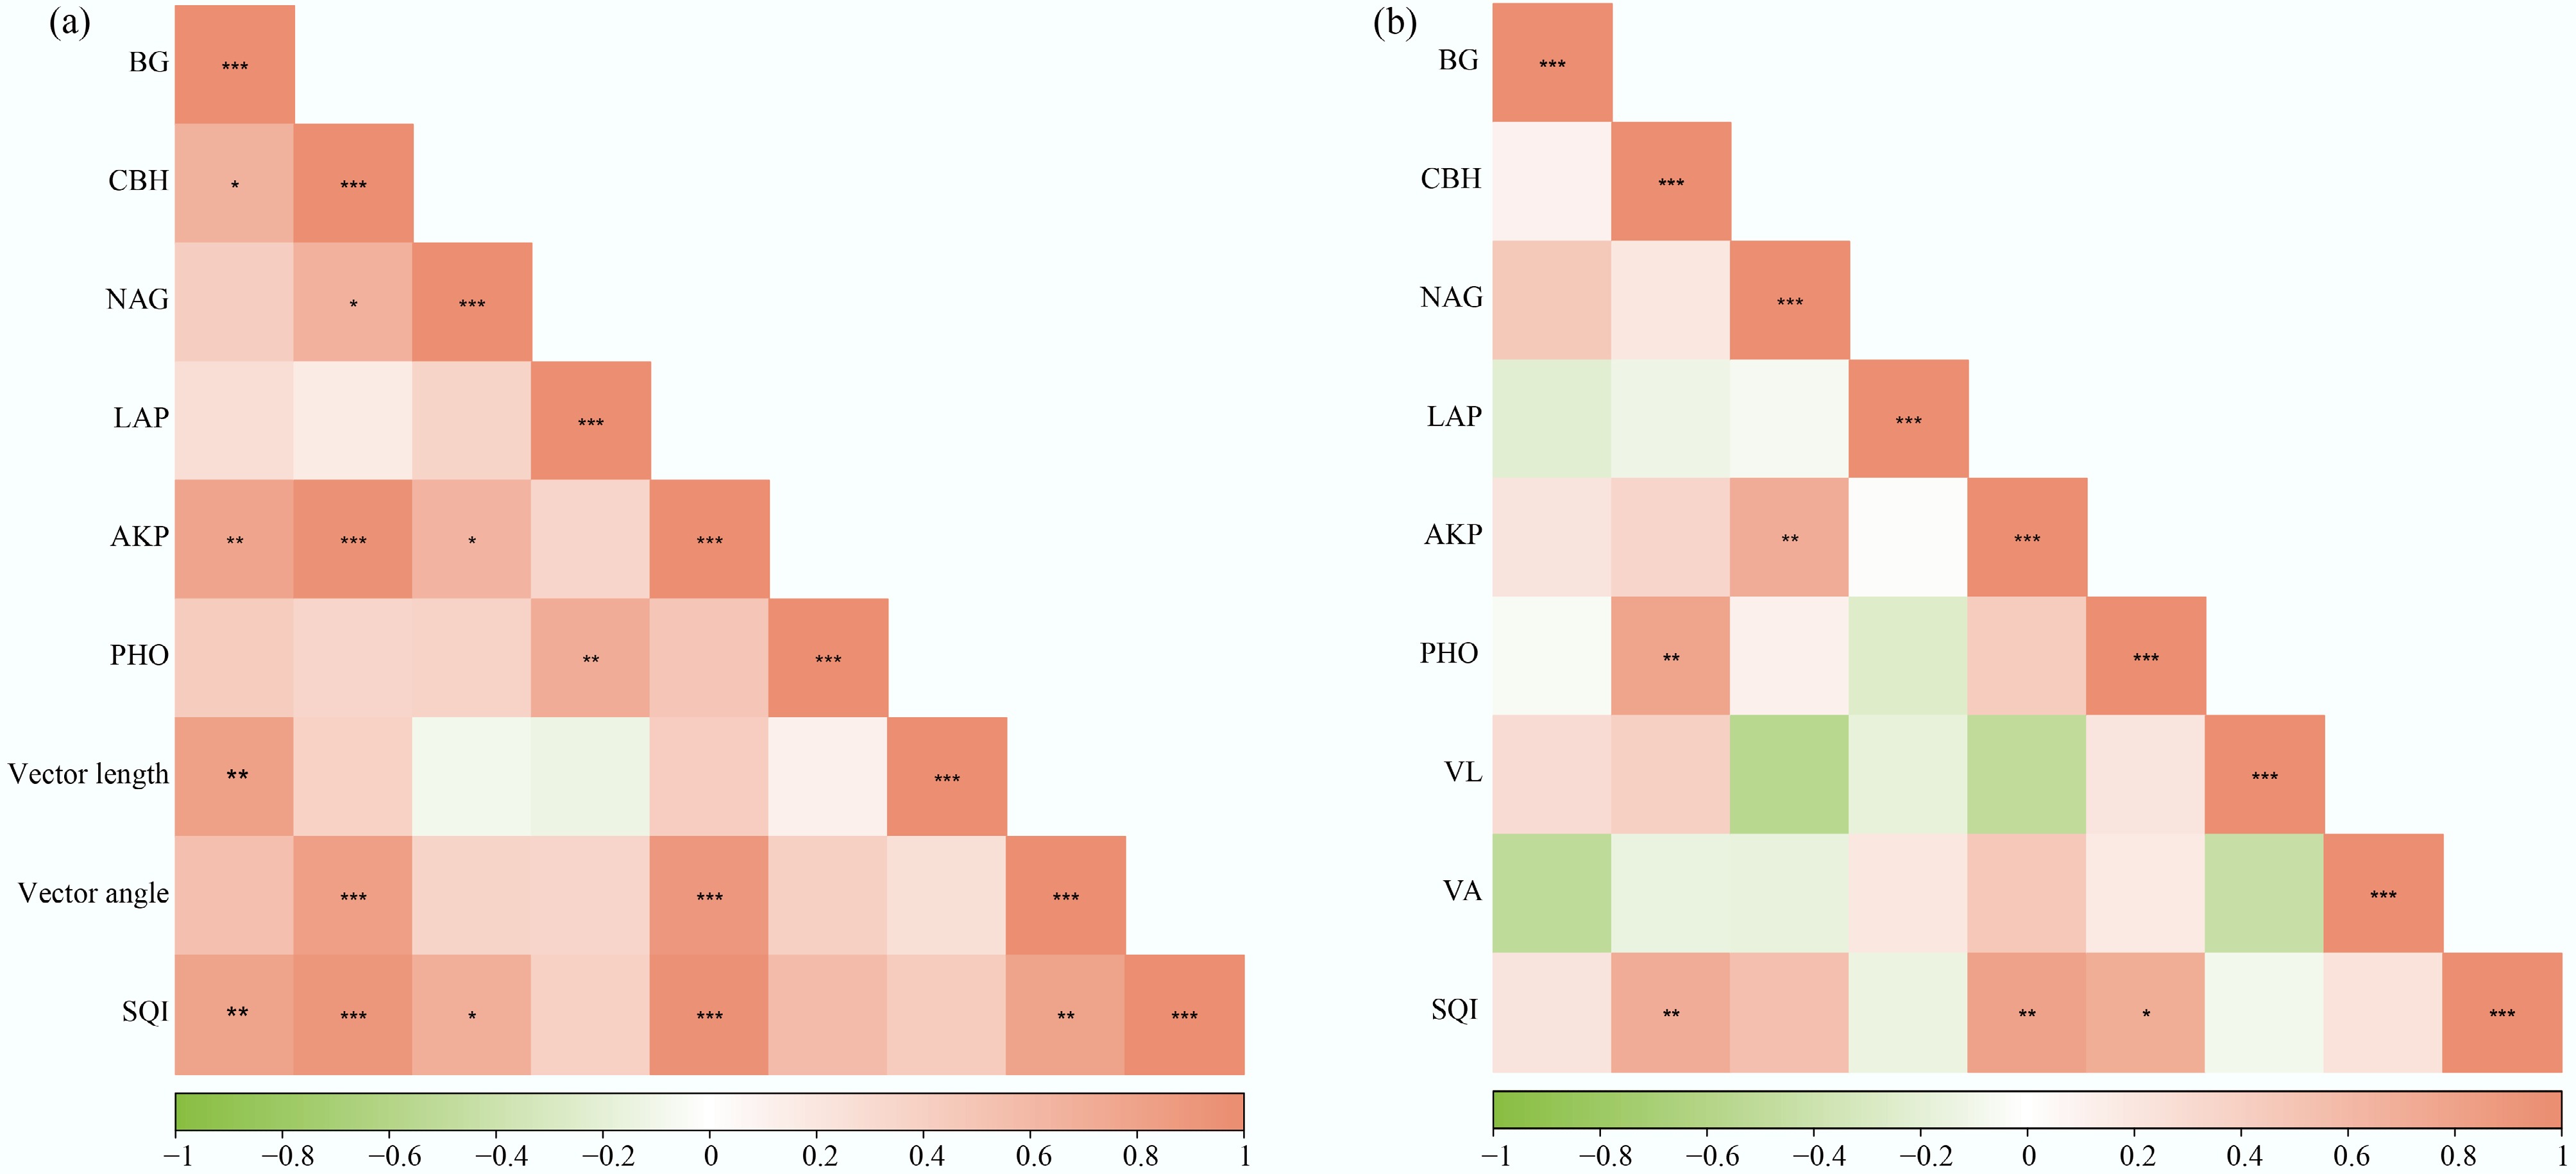
Figure 6.
Correlation analysis between soil quality index and extracellular enzyme activities in the (a) topsoil (0–20 cm), and (b) subsoil (20–40 cm). BG, β-glucosidase; CBH, cellobiosidase; NAG, β-N-acetyl-glucosaminidase; LAP, L-leucine aminopeptidase; AKP, alkaline phosphatase; PHO, phenol oxidase. *** p < 0.001; ** p < 0.01; * p < 0.05.
-
Consistent with the initial hypothesis, long-term SW markedly increased SOC and TN stocks in the topsoil (Fig. 1). These increases were closely associated with a synergistic mechanism between aggregate formation and microbial activity[14]. By enhancing soil nutrient availability, SW stimulated microbial growth and the production of extracellular polymeric substances and fungal hyphae, which act as binding agents for soil particle aggregation. The resulting increase in macroaggregate formation provided physical protection for SOC by limiting direct contact between SOC and microorganisms, thereby suppressing microbial decomposition[19,35]. In turn, the enhanced SOC availability further promoted microbial activity, creating a positive feedback loop that reinforced aggregate stability and SOC sequestration[8,36,37]. This process further promoted the transformation of labile SOC fractions (e.g., DOC, MBC) into more recalcitrant C forms, contributing to long-term C stabilization[38]. However, there were no significant variations in subsoil SOC stocks across all treatments (Fig. 1). This lack of significance could be associated with no-tillage combined with wheat straw retention, which may have resulted in the predominant accumulation of residues in the topsoil. Moreover, crop roots are mainly distributed in the topsoil[39,40], and the organic compounds released by roots are also predominantly concentrated in the surface soil layer. Notably, subsoil TN stock under SW was the highest among all treatments and significantly higher than that under MW (Fig. 1). This phenomenon may be related to the downward transport of N from the topsoil (e.g., via nitrate leaching into the subsoil)[41], and may also be influenced by the contrasting residue inputs and root characteristics inherent to the different cropping systems.
Enzyme activities and stoichiometries
-
Compared with MW and CW rotations, SW markedly enhanced the activities of C- and P-acquiring enzymes (Fig. 2), which is in line with the second hypothesis. SW facilitates the improvement of soil aggregate structure, constructing a suitable microhabitat for the proliferation of soil microbial communities[42]. The enhanced soil N availability under SW may promote microbial growth and metabolism, thereby increasing microbial C demand and utilization[26,43]. The enhancement in soil MBC and MBN contents also confirms this conclusion (Fig. 1j, k). In addition, the relatively sufficient available N content under SW can stimulate microbial P demand, thereby promoting the synthesis of P-acquiring enzymes to meet the normal metabolic needs of microorganisms[44,45]. Compared with maize and cotton, soybean has a higher inherent demand for P[46], which not only further drives the increase in soil C-acquiring enzyme activities, but also stimulates the release of greater amounts of low molecular weight organic acids in its rhizosphere to reduce soil pH, thereby converting recalcitrant P fractions in the rhizosphere into available forms[24,46]. Research indicates that leguminous crops can secrete organic acids and phosphatases to activate insoluble P in the soil and convert it into plant-available forms for absorption and utilization[44,47]. Soil enzyme activity declined with deepening of the soil layer, which was consistent with the declining trends in soil microbial activity and nutrient availability along the soil layer (Fig. 2). This was primarily because the topsoil of farmland serves as the main active zone for crop roots and microorganisms, and enzyme synthesis is regulated by soil resource limitation[8,19].
From the perspective of soil enzyme stoichiometry, all treatments in this study showed a consistent pattern of higher relative investment in P acquisition (vector angle > 45°), with the vector angle under SW markedly higher than those under MW and CW in the topsoil (Fig. 3c). This pattern was closely related to the inherent alkaline nature of the tested soil (pH > 8.0): compared with neutral soils, P in alkaline environments readily combines with calcium to form insoluble calcium phosphate complexes, which markedly reduces the bioavailability of soil P and may contribute to greater microbial P demand[48,49]. Additionally, soybean has a higher inherent P demand than maize and cotton[46], which may further increase soil P consumption and is associated with a higher vector angle under SW than under MW and CW. Wang et al.[27] reported that SW significantly increased functional genes (e.g., phoD) associated with soil organic P mineralization. This reflects the adaptive strategy of microorganisms in response to P limitation, i.e., regulating the expression of genes involved in P mineralization to satisfy P demand. Notably, SW increased AP while also exhibiting a higher vector angle (Figs 1f, 3c). This suggests that microbial P demand increased disproportionately relative to C and N demand, likely driven by enhanced microbial growth and activity under SW. By contrast, vector length did not differ significantly among the treatments (Fig. 3), indicating that the relative investment in C acquisition was comparable across different rotation systems. This phenomenon may be due to the continuous supply of labile C substrates to the soil through wheat straw returning, thus minimizing differences in soil C availability. However, vector length in the topsoil was significantly greater than that in the subsoil, aligning with earlier findings[8,11]. The main reason is that the topsoil serves as the core zone for microbial colonization and metabolism, where higher microbial activity and C consumption rates lead to greater relative investment in C acquisition compared with the subsoil[11].
Factors mediating soil quality
-
Soil quality reflects the integrated capacity of an ecosystem to support biodiversity, drive nutrient cycling, and improve crop productivity[10,50]. Compared with MW and CW, SW significantly increased the SQI in both topsoil and subsoil layers (Fig. 4). This was primarily driven by greater SOC and TN stocks and higher nutrient availability under SW, which provided more nutrients and energy for soil microorganisms, promoted nutrient cycling, and consequently improved the SQI[8]. In addition, higher nutrient availability enhanced microbial activity and stimulated soil enzyme secretion, creating hotspots of microbial activity[51,52]. These hotspots play critical roles in regulating nutrient utilization and maintaining soil quality[11,19]. The higher soil N availability under SW may stimulate microbial demand for C and P, promote the synthesis of C- and P-acquiring enzymes, and further accelerate soil nutrient cycling. Correlation analysis also revealed that SQI was markedly positively correlated with C- and P-acquiring enzymes (Fig. 6). Especially in the topsoil, higher BG and CBH accelerated wheat straw decomposition and enhanced DOC content, whereas elevated AKP activity increased AP supply. These improvements in nutrient availability and cycling efficiency ultimately enhanced soil quality[53,54]. Collectively, sufficient C, N, and P supply favored the growth and reproduction of diverse microbes, accelerated biogeochemical cycling, and improved SQI[50,55,56]. The positive correlation between vector angle and SQI also provided additional evidence for this association (Fig. 5).
Overall, SW shows potential for improving soil quality in both the topsoil and subsoil layers. However, P demand increased under this rotation system, and the tested soil is alkaline, where P is readily fixed into unavailable forms. Therefore, applying additional P fertilizer, using physiologically acidic P fertilizers (e.g., monoammonium phosphate), or combining P fertilizer with organic amendments may help enhance P availability.
Limitations
-
Despite the comprehensive insights provided by this study regarding the effects of SW on soil quality and extracellular enzyme stoichiometry, certain constraints of this study warrant acknowledgment. First, soil sampling was conducted only once; repeated sampling over multiple years would provide a more comprehensive understanding of the long-term impact of the rotation system on soil quality. Future research should incorporate continuous monitoring and data collection across multiple seasons. Second, this study measured soil properties only in the 0–40 cm soil layer, which may underestimate potential changes in deeper soil layers. Future studies should include assessment of deeper soil layers. Third, this study compared the overall effects of the complete rotation system, without separately isolating the biological N fixation effect of soybean or evaluating indicators such as crop yield, N loss, and economic benefits. This limitation restricted the assessment of the comprehensive benefits of SW. Future research should combine long-term site-specific monitoring, deep soil analysis, and multi-dimensional ecosystem indicator assessment to more comprehensively evaluate the SW system.
-
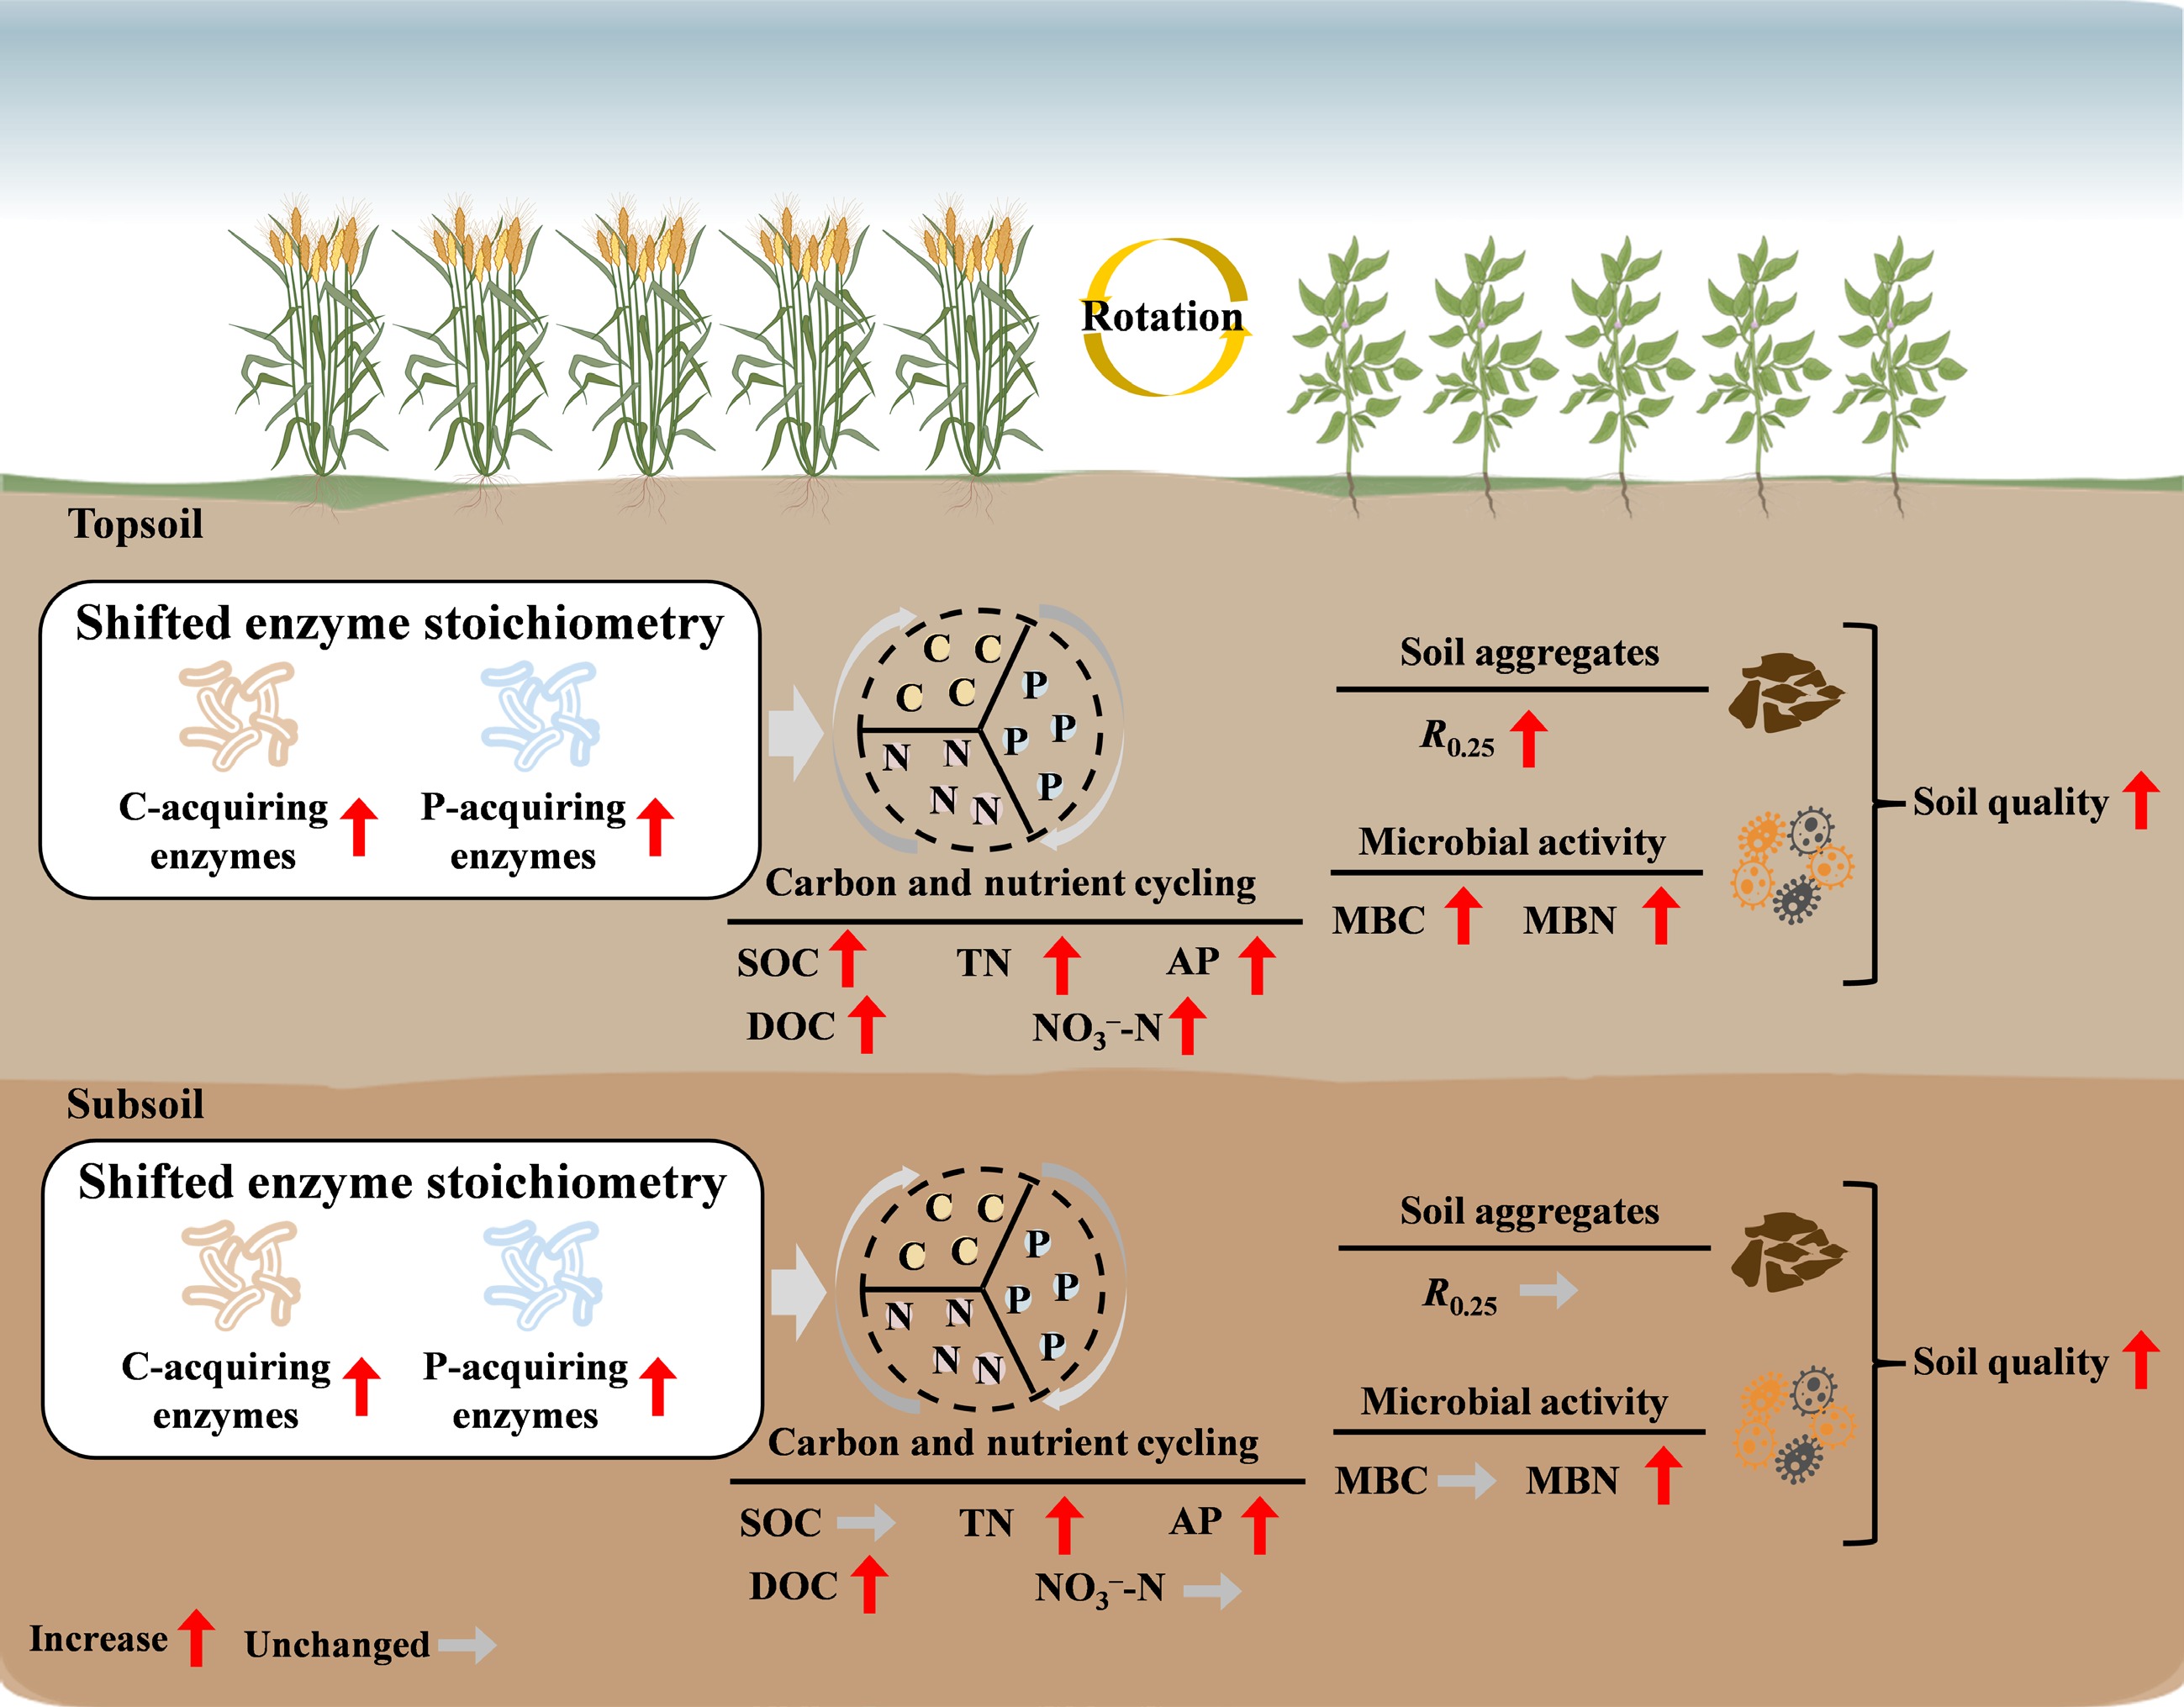
This study demonstrated that SW significantly increased topsoil SOC and TN stocks while also enhancing the activities of C- and P-acquiring extracellular enzymes in both the topsoil and subsoil. SW significantly improved the SQI in both the topsoil and subsoil, which was closely associated with C- and P-acquiring enzyme activities. In addition, P fertilizer application should be appropriately increased to meet the higher P demand under this rotation system. Under alkaline soil conditions, the use of physiologically acidic P fertilizers or combined application with organic amendments is recommended to enhance P availability. Overall, SW shows potential for improving soil quality within the 0–40 cm layer, but its long-term sustainability and broader applicability require further assessment incorporating crop yield, N losses, and economic benefits.
No acknowledgements are applicable for this work.
-
It accompanies this paper at: https://doi.org/10.48130/nc-0026-0017
-
Not applicable.
-
The authors confirm their contributions to the paper as follows: Quanyi Hu: writing – original draft, project administration, funding acquisition; Guangshuai Wang: resources; Fangting Guo: validation, investigation; Yali Zhao: supervision, formal analysis; Tianqi Liu: writing – review & editing; Peter D. Kemp: writing – review & editing; Yingxin Xie: writing – review & editing, conceptualization; Xuelin Zhang: writing – review & editing, conceptualization. All authors reviewed the results and approved the final version of the manuscript.
-
The data generated and analyzed during the current study are not publicly archived but can be obtained by the corresponding author upon reasonable request.
-
The authors declare that they have no conflict of interest.
-
Full list of author information is available at the end of the article.
- The supplementary files can be downloaded from here.
- Copyright: © 2026 by the author(s). Published by Maximum Academic Press, Fayetteville, GA. This article is an open access article distributed under Creative Commons Attribution License (CC BY 4.0), visit https://creativecommons.org/licenses/by/4.0/.
-
About this article
Cite this article
Hu Q, Wang G, Guo F, Zhao Y, Liu T, et al. 2026. Long-term soybean–wheat rotation improves soil quality and shifts extracellular enzyme stoichiometry. Nitrogen Cycling 2: e030 doi: 10.48130/nc-0026-0017 
Long-term soybean–wheat rotation improves soil quality and shifts extracellular enzyme stoichiometry
- Received: 08 July 2026
- Revised: 05 September 2026
- Accepted: 09 October 2026
- Published online: 02 November 2026
Abstract: Legume-based rotation is a sustainable cropping system that can effectively improve soil fertility. However, systematic studies and evaluations of its long-term effects on soil quality across different soil layers remain limited. In a 14-year field trial on the Huang-Huai-Hai Plain, we evaluated soil organic carbon (SOC), total nitrogen (TN), extracellular enzyme stoichiometry, and soil quality index (SQI) across three rotation systems: soybean–wheat rotation (SW), maize–wheat rotation (MW), and cotton–wheat rotation (CW). Results indicated that SW significantly enhanced SOC and TN stocks, dissolved organic carbon, nitrate N, available phosphorus (AP), and microbial biomass C and N in the topsoil (0–20 cm) compared to MW and CW, while also increasing TN, AP, and microbial biomass N in the subsoil (20–40 cm). SW significantly increased the activities of C- and P-acquiring enzymes in both soil layers. Enzyme stoichiometry indicated a higher relative investment in P acquisition across all treatments, with SW showing a significantly greater vector angle, suggesting a potential increase in relative demand for P. Notably, SW markedly increased SQI by 30.0%–36.7% in the topsoil and 18.5%–24.3% in the subsoil compared with MW and CW. The correlation analysis indicated a strong association between SQI and the activities of soil C- and P-acquiring enzymes. Overall, SW markedly enhanced soil nutrient status, extracellular enzyme activities, and soil quality in both the topsoil and subsoil, though it was also associated with higher P demand. These results provide empirical support for optimizing cropping systems and improving soil quality in intensive agricultural regions.