










-
Tea, one of the world's most popular beverages, is primarily manufactured from the young shoots of the tea plant (Camellia sinensis [L.] O. Kuntze)[1]. Its distinctive flavor and health benefits are directly attributed to key secondary metabolites, including theanine (contributing to a umami taste), catechins (responsible for astringency), caffeine (imparting bitterness), and diverse volatile compounds (forming complex aromas)[2,3] (Fig. 1). The balance of these components ultimately defines tea quality and market value.
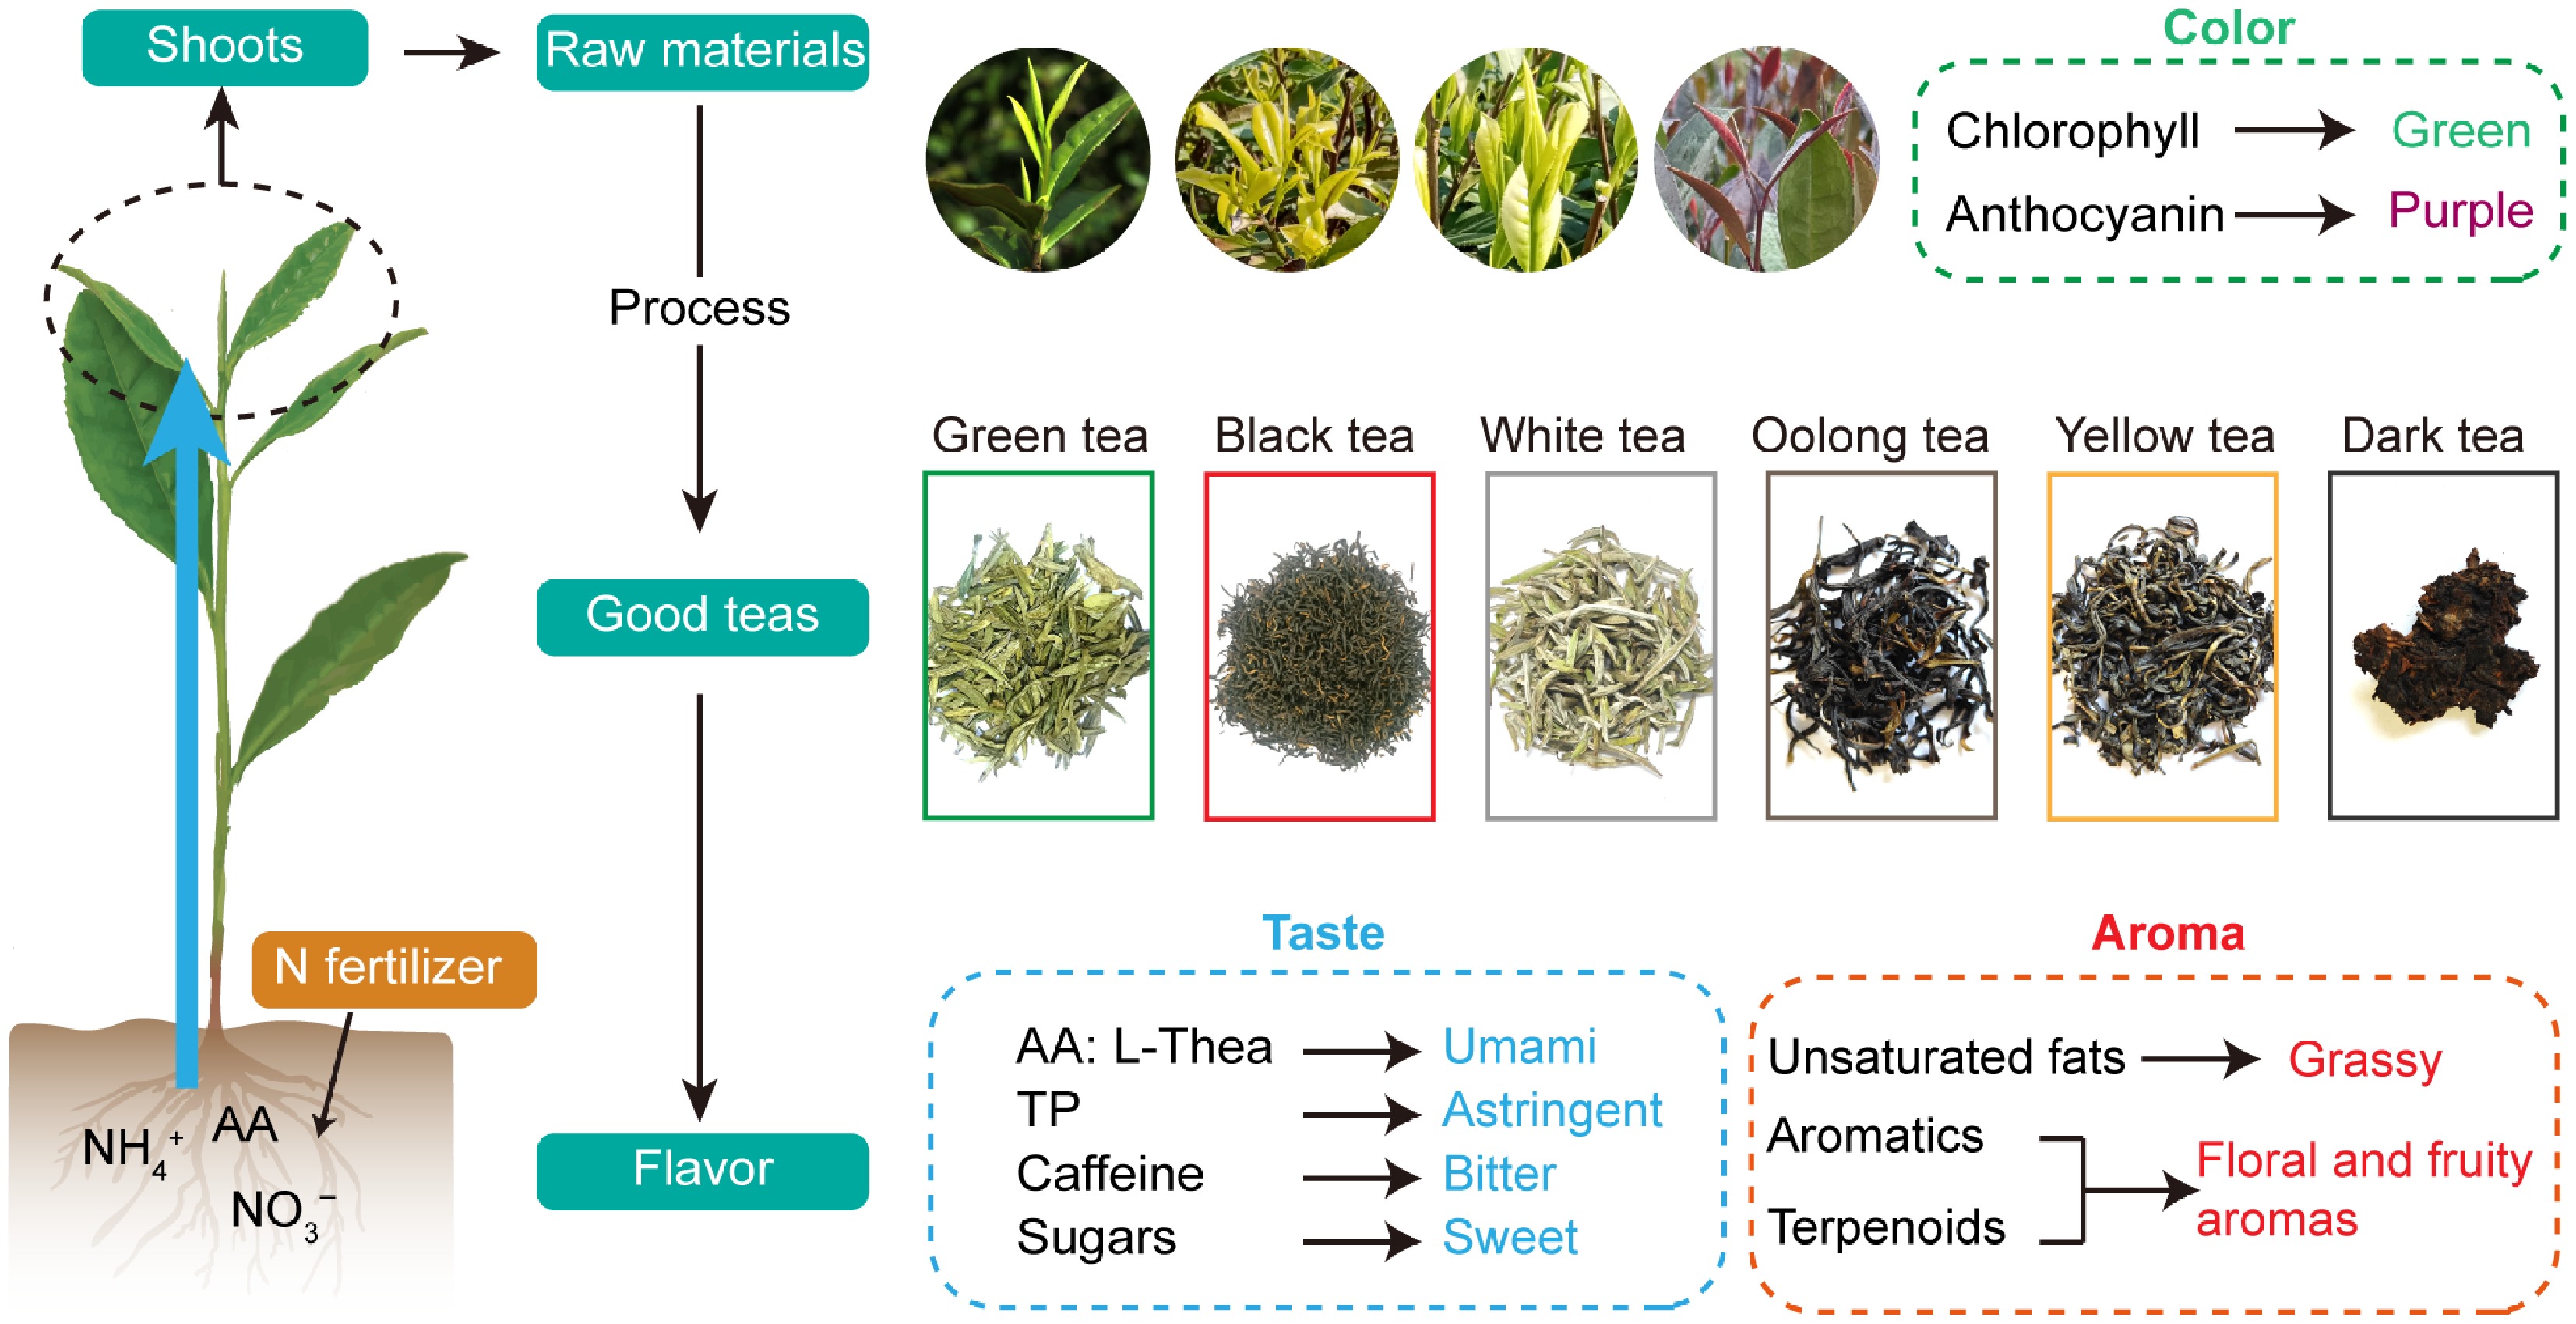
Figure 1.
N application levels and forms regulate the secondary metabolites in fresh tea shoots and dictate tea sensory quality. N application levels and forms (e.g., NH4+, NO3−, amino acids) directly shape the metabolic profile of new tea plant shoots, with the balance of key metabolites determining their processing suitability for specific tea types. These metabolites collectively define tea flavor: theanine imparts umami and sweetness, catechins contribute bitterness and astringency, caffeine enhances a bitter aftertaste, and diverse volatile compounds form a complex aroma profile. Abbreviations: AA, amino acids; TP, tea polyphenols.
In modern tea cultivation, N fertilization is a fundamental agronomic practice to ensure high yields[4]. However, the relationship between N supply and tea quality is not straightforward. Excessive and improper N application has become a widespread issue, frequently leading to a decline in quality (such as reduced aroma complexity and an imbalance between umami and astringency)[5,6], while also causing low NUE, soil acidification, and environmental concerns[7−9]. Therefore, moving beyond simple yield-based fertilization towards quality-oriented N management is a critical challenge for the sustainable and profitable development of the tea industry.
This review synthesizes current knowledge on how N regulates the biosynthesis and accumulation of these key quality-determining metabolites in tea plants. We summarize the specific effects of N forms and doses on theanine, catechins, caffeine, and aroma substances. Furthermore, we discuss the practical implications of N-mediated metabolic crosstalk for quality formation. Finally, we explore future strategies centered on optimizing N management and breeding new tea varieties, with the dual goals of enhancing tea quality and improving NUE for a more sustainable tea industry.
-
Theanine is a unique non-proteinogenic amino acid that defines the umami taste, and serves as a major N storage compound in tea plants[9,10]. Its metabolism is spatially separated between roots and shoots. Biosynthesis occurs predominantly in the roots, where theanine synthase (CsTSI) conjugates ethylamine (derived from alanine by CsAlaDC), and glutamate (synthesized via CsGDH or CsGOGAT)[9,11] (Fig. 2a).
N regulates theanine biosynthesis and store in roots
-
N availability directly controls the start of the pipeline—theanine synthesis in roots. Theanine accumulation increased under elevated N concentrations to some extent[5,12,13]. The form of N is also critical; ammonium (NH4+) and its precursor ethylamine are consistently more effective than nitrate (NO3−) at stimulating theanine accumulation[14−16] (Fig. 2b, c). This preference underscores the importance of selecting ammonium-based fertilizers in tea garden management to enhance the umami taste.
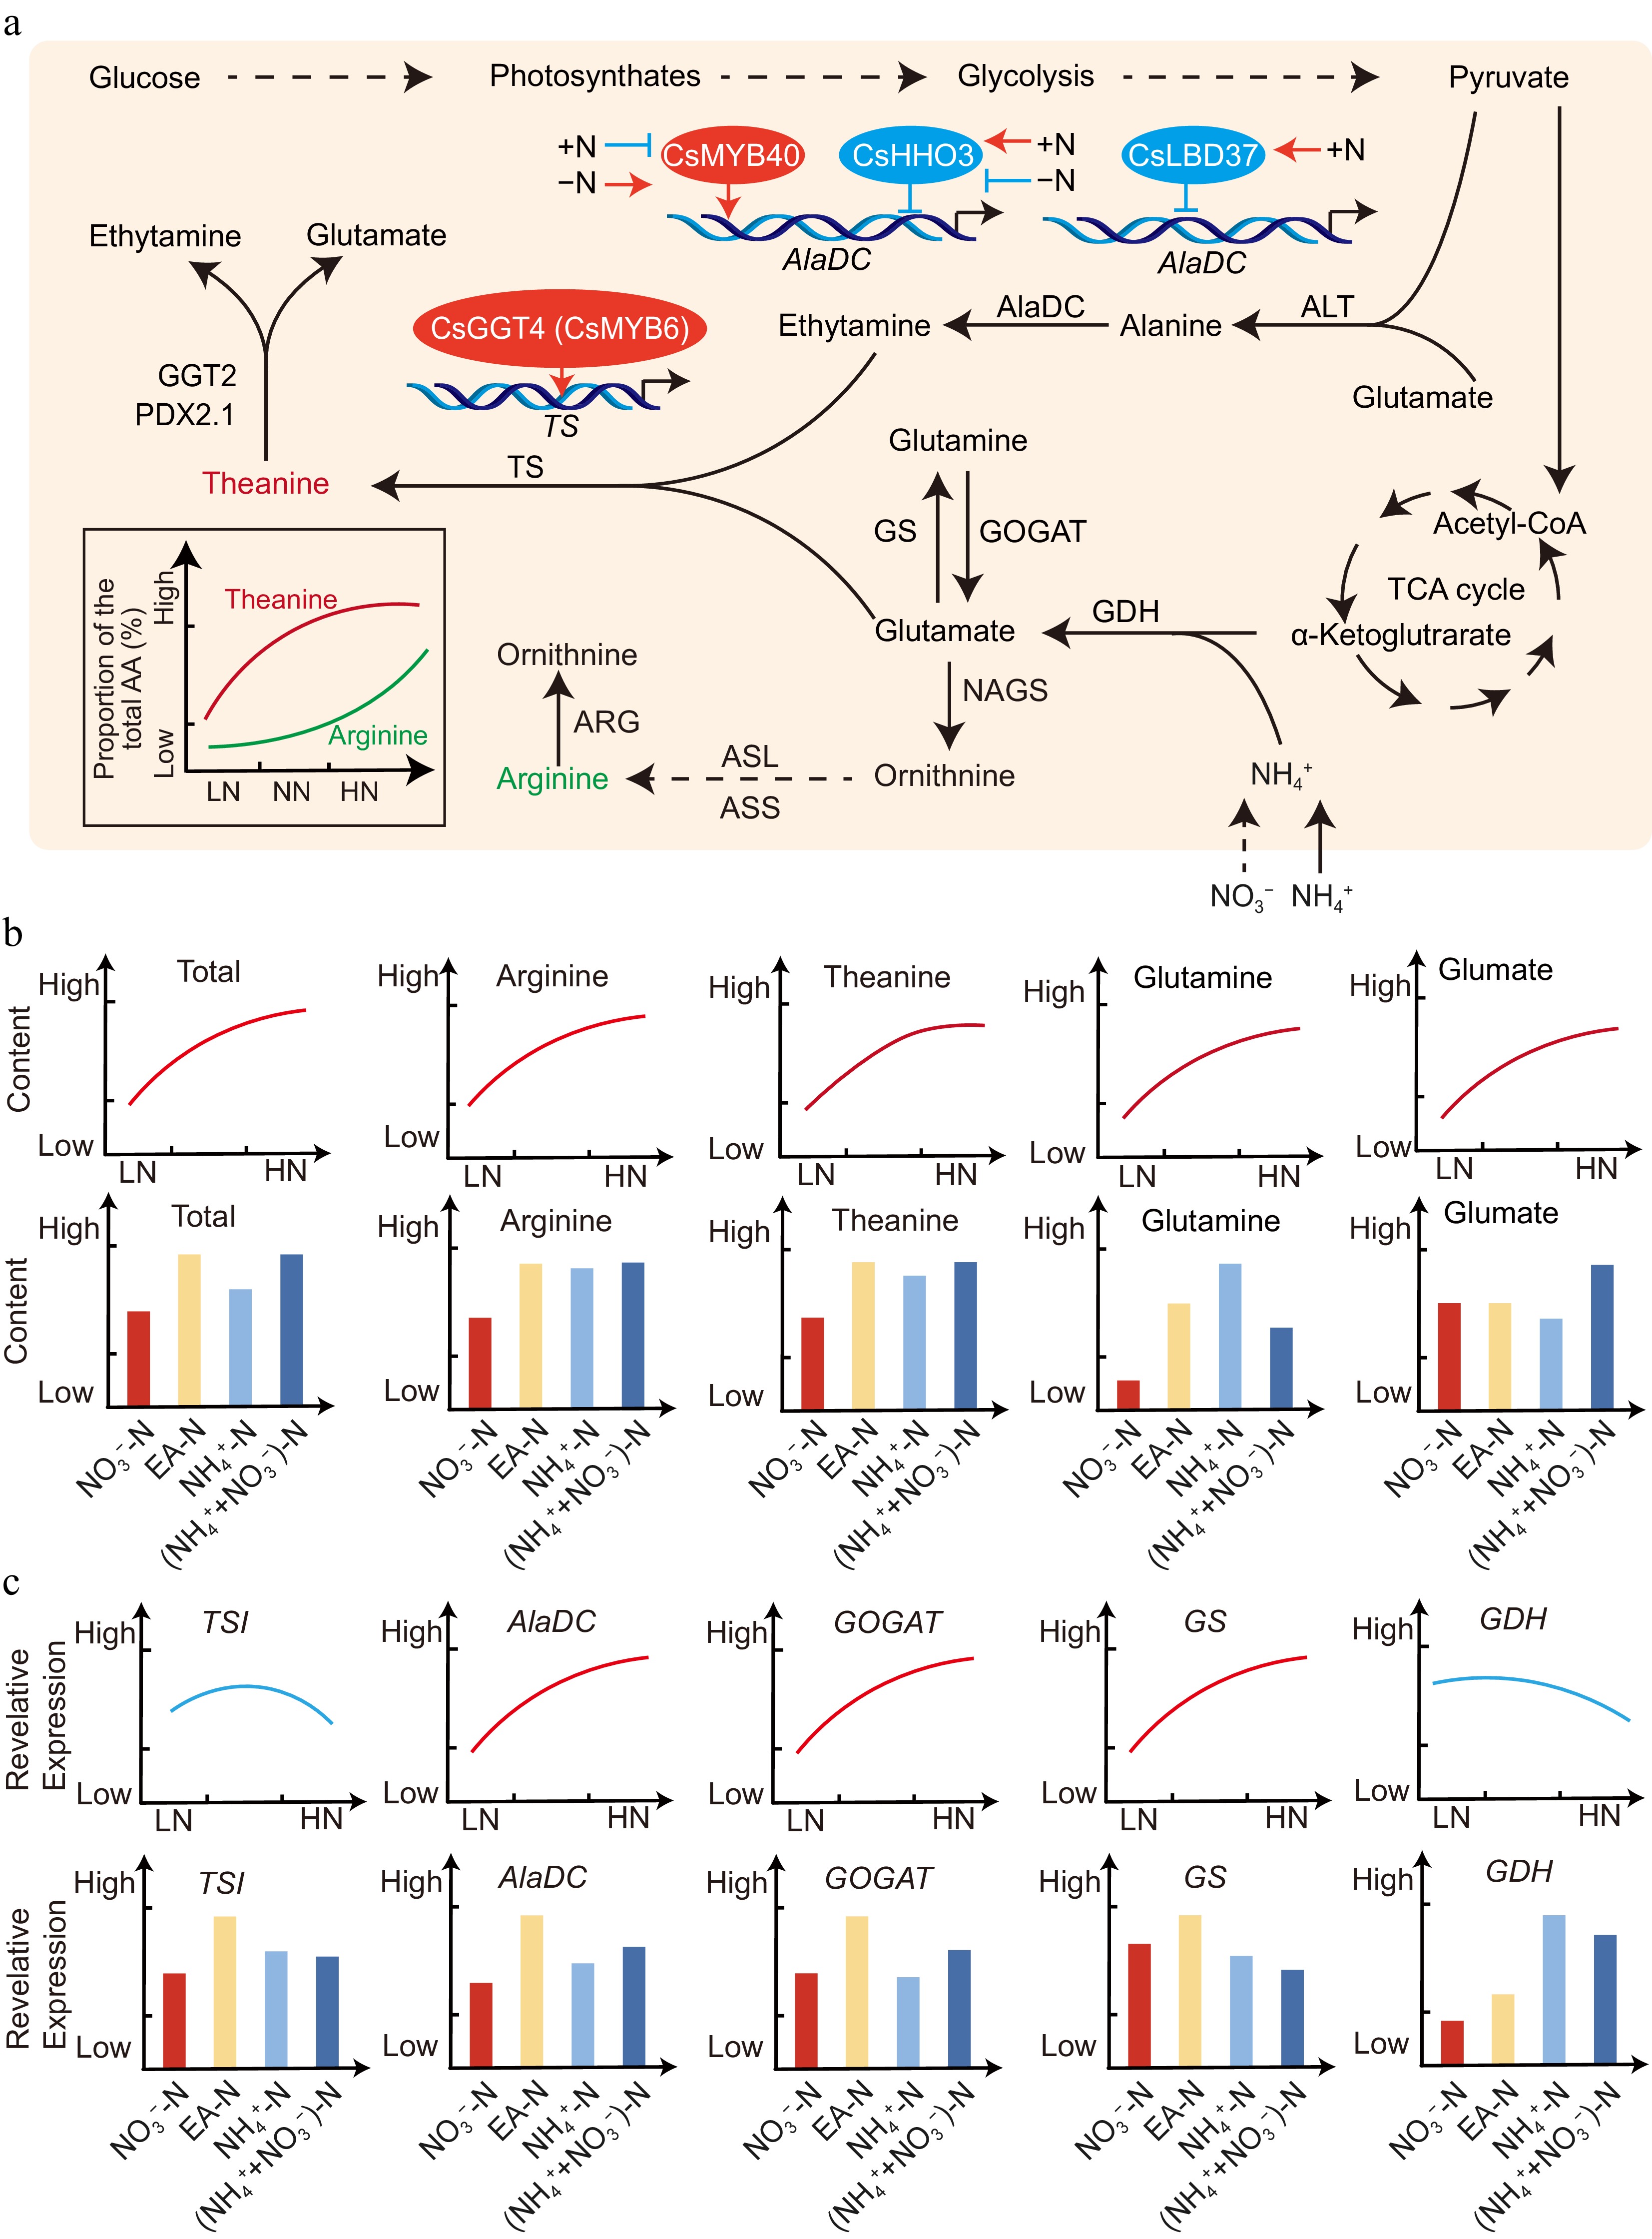
Figure 2.
N regulates amino acid biosynthesis and accumulation in tea plants. Different N levels, and forms, regulate the biosynthesis and subsequent accumulation of amino acids. The proportion of arginine to total amino acids in tea increased significantly with increasing N application, while theanine decreased. In addition, theanine accumulation is regulated at the transcriptional level. CsHHO3 and CsLBD37 inhibited CsAlaDC expression under high N, and CsMYB40 induced CsAlaDC expression under low N[16−19]. (a) Amino acid content under different N levels and forms; (b) relative expression under different N levels and forms, and (c) N regulates amino acids accumulation. Abbreviations: HN, high N level; LN, low N level; NN, normal N level.
This response is mediated by the transcriptional regulation of key biosynthetic genes. The expression of CsAlaDC shows a strong positive correlation with theanine content and is regulated by specific transcription factors in response to N status[20,21]. The expression of CsAlaDC, which is strongly correlated with theanine content, is finely modulated by a network of transcription factors in response to N status. Under high N, repressors like CsHHO3 and CsLBD37 act as 'brakes' to downregulate CsAlaDC, preventing potential over-accumulation. In contrast, low N conditions induce potential activators like CsMYB40, which may function as an 'accelerator'[13,22] (Fig. 2a). This sophisticated regulation highlights that simply applying more N is not always better; the goal is to maintain an optimal level that maximizes synthesis, without triggering these repressive mechanisms.
N regulates theanine accumulation and catabolism in tea plant shoots
-
Theanine concentration in tea shoots is a net result of its biosynthesis in roots, transport to shoots, and catabolism within shoots. Hydrolysis back to glutamate and ethylamine is likely catalyzed by enzymes such as CsPDX2.1 or CsGGT2, releasing N for use in leaf growth and metabolism[23,24] (Fig. 2a). The system is fine tuned by transcription factors like CsMYB73, which simultaneously promotes catabolism (via CsGGT2) and inhibits a shoot-based synthesis pathway (via CsGGT4), ensuring dynamic control over the final theanine pool in harvested shoots[25]. N availability influences all these processes, including catabolism in new shoots. Generally, theanine levels in leaves and roots show similar trends in response to different N levels and forms[5,14,26,27]. For instance, the expression of the catabolic gene CsPDX2.1 is lowest under low N, potentially as a conservation strategy, and shifts under different N sufficiency levels[5]. This suggests that N management can influence not just the supply of theanine, but also its retention in the leaf. Optimizing N application to minimize catabolism in the shoot could be a novel strategy to further boost theanine accumulation.
Interactive effects of N with other nutrients on theanine
-
The effect of N on theanine is modulated by interactions with other nutrients, underscoring the importance of balanced fertilization. Other nutrients interact with N to modulate theanine metabolism. Magnesium (Mg) plays a vital role by promoting both theanine biosynthesis in roots and its long-distance transport to shoots[28,29]. As a cofactor for many enzymes, Mg is essential for the energy-intensive processes of synthesis and phloem loading.
Similarly, appropriate application of potassium (K) fertilizer increases theanine content while decreasing arginine levels[30,31]. This may be attributed to the role of K in altering N storage forms. Therefore, achieving high theanine levels is not just about N fertilizer; it requires an integrated nutrient management approach that includes adequate Mg and K to ensure efficient N utilization and translocation.
N regulates theanine transport
-
After synthesis, theanine is transported to new shoots through the vascular system[26,32]. This long-distance transport relies on a suite of amino acid transporters that orchestrate xylem loading in roots, xylem-to-phloem transfer in stems, and finally phloem unloading into sink tissues (new shoots)[26,33,34]. Efficient transport from root to shoot is essential for delivering theanine to the commercially valuable tender shoots. This process is mediated by specific CsAAP transporters, each with distinct tissue expression patterns, suggesting specialized roles in loading, transfer, and unloading. Crucially, the expression of many of these transporters is induced by N deficiency, indicating a plant strategy to enhance N retrieval and mobilization under scarcity[26,33,35].
For instance, CsAAP1 expression in roots correlates with root-to-shoot theanine translocation, marking it as a key candidate for improving N distribution[26]. Similarly, CsAAP7.2 has been shown to be essential for the long-distance transport of theanine[34] (Fig. 3). Recent studies highlight that inhibiting the theanine transporter CsCAT1, or the mitochondrial transporter CsTHS1, can increase theanine retention in young leaves, offering potential strategies for flavor enhancement[36,37]. These transporters represent potential breeding targets for developing tea cultivars that more efficiently allocate theanine to the shoots, thereby improving quality without increasing fertilizer input.
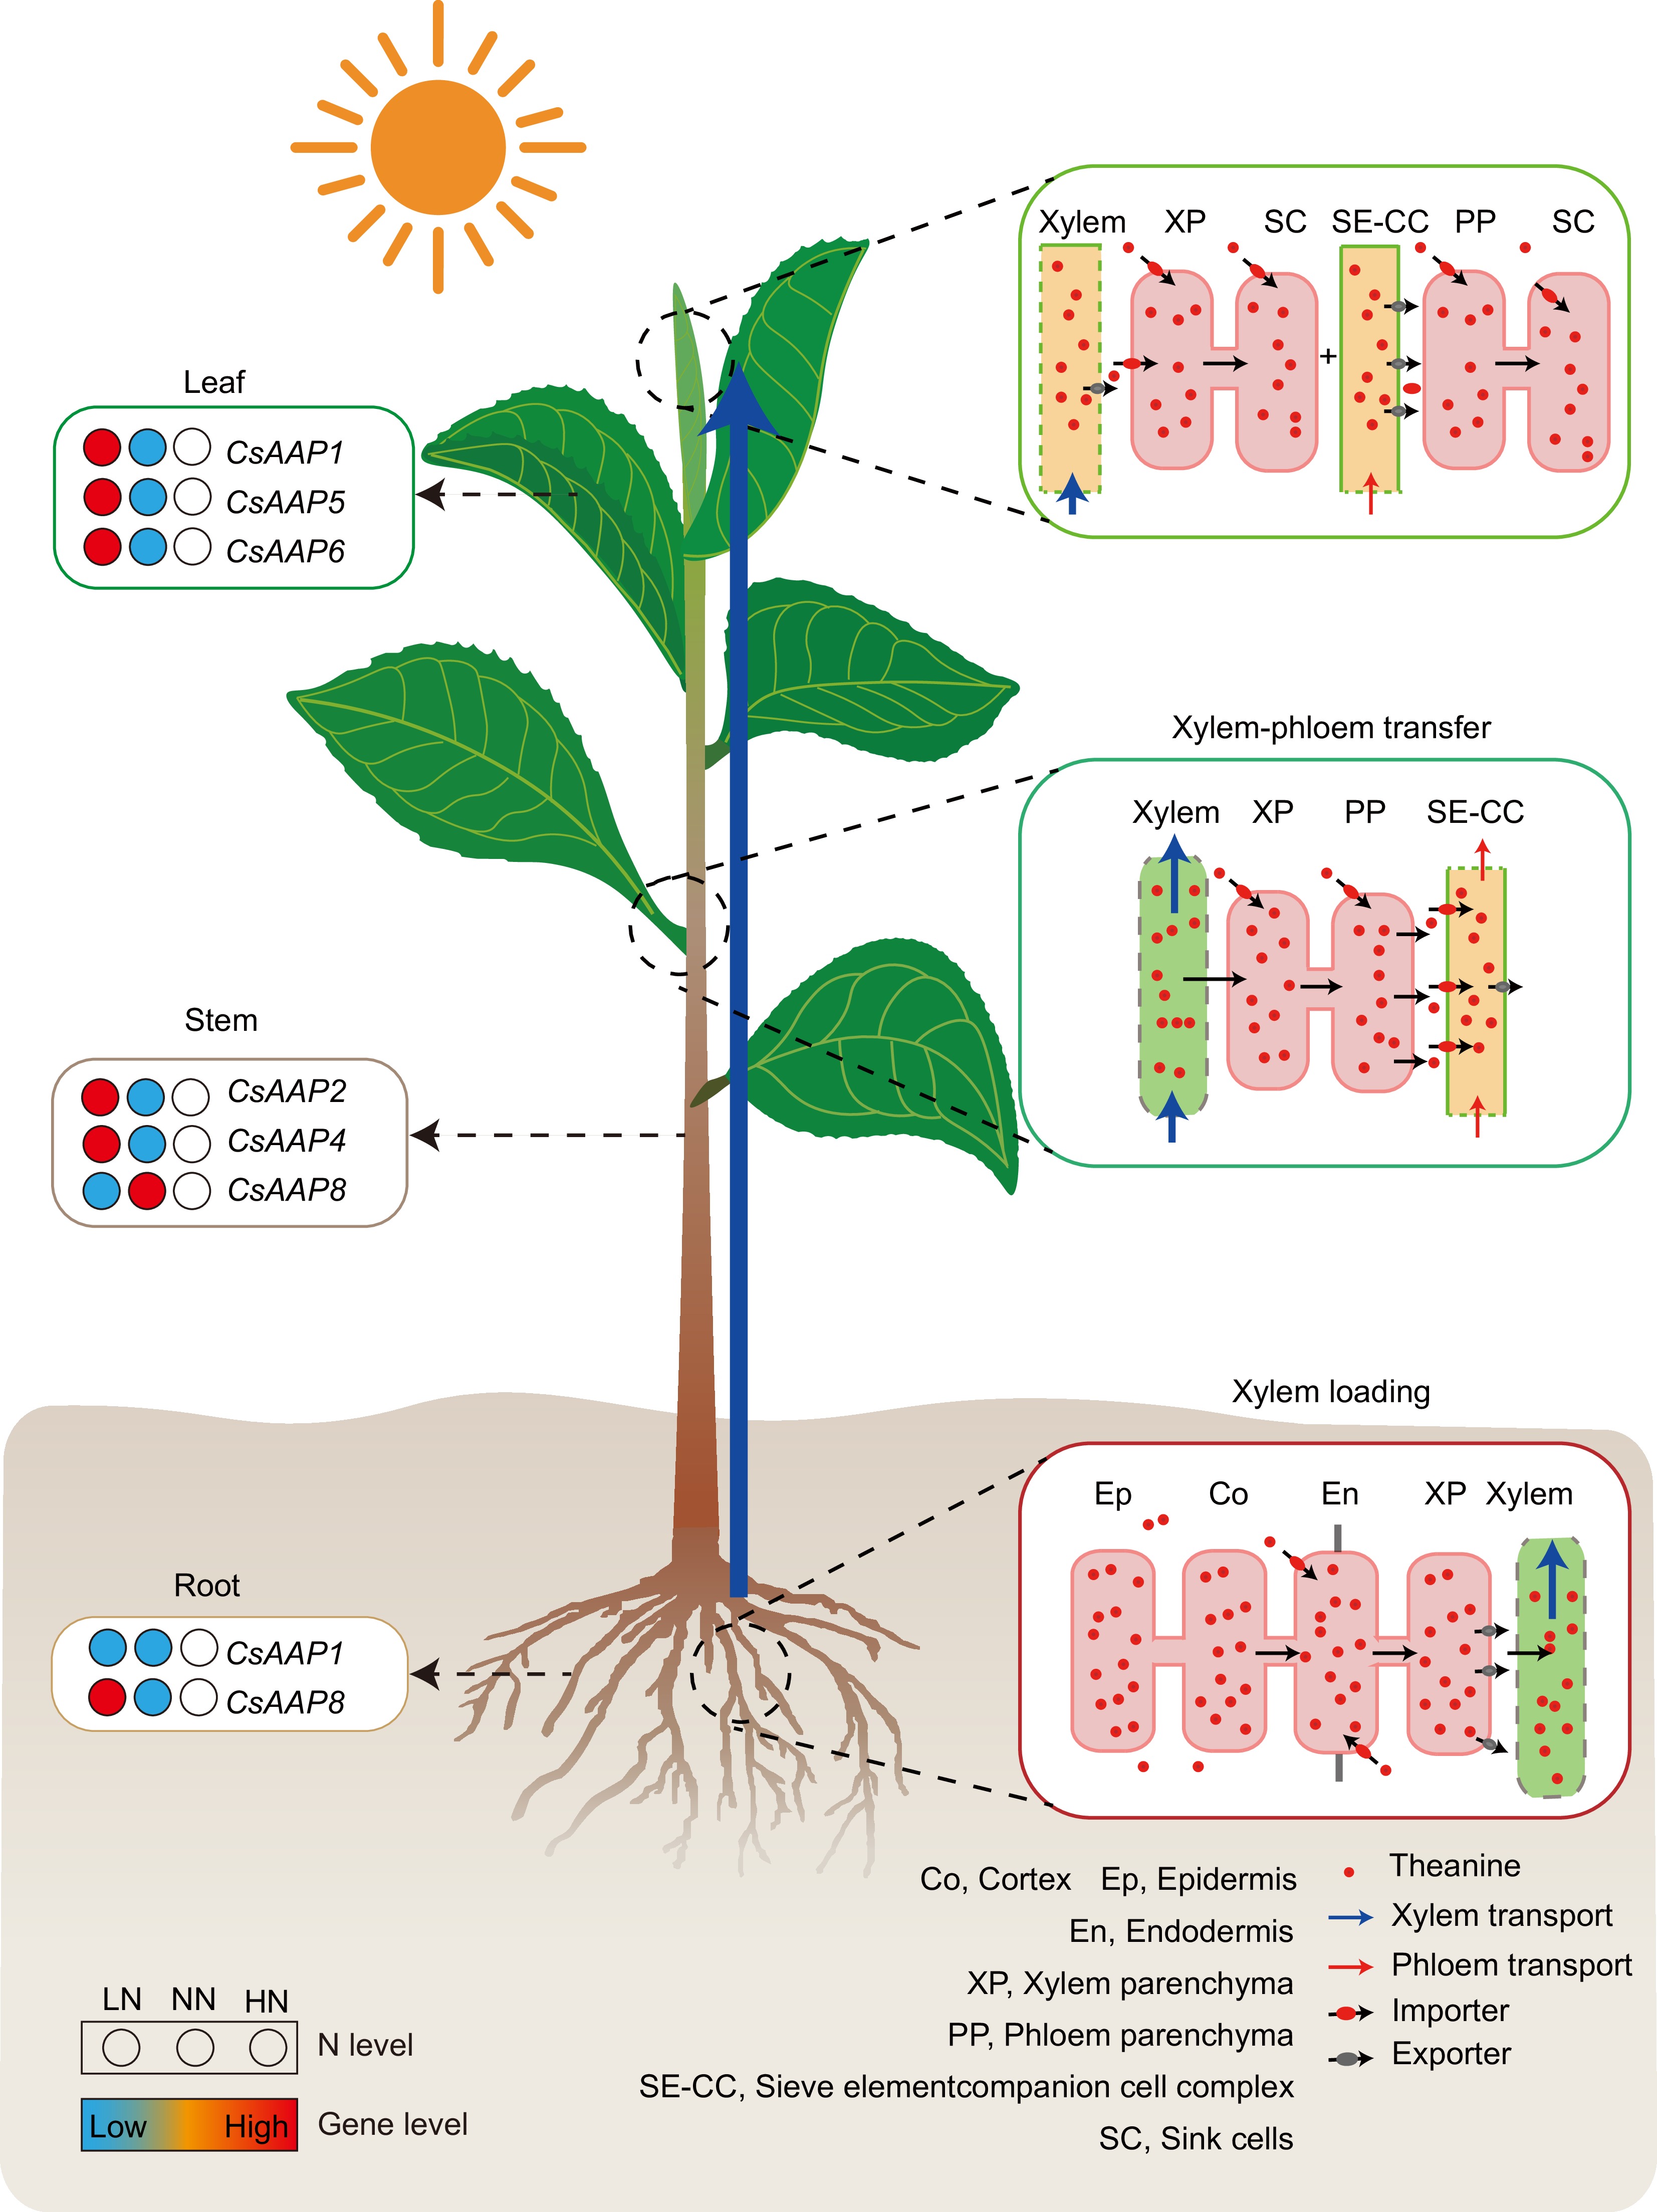
Figure 3.
N regulates theanine transport. The theanine transport pathway in tea plants proceeds sequentially through xylem loading, xylem-to-phloem transfer, and phloem unloading into the apoplasmic space adjacent to the sieve element-companion cell complex, followed by final delivery to new shoots. The expression profiles of specific amino acid transporters (CsAAPs) are annotated for each cell type using a color gradient (blue: low expression; red: high expression), highlighting their regulatory roles in mediating these xylem loading, xylem-to-phloem transfer, and phloem unloading steps under varying N levels[22,32,33]. Abbreviations: HN, high N level; LN, low N level; NN, normal N level.
-
A high concentration of polyphenols, particularly catechins, in new shoots is a defining biochemical characteristic of the tea plant. Catechins, which account for approximately 80% of the total polyphenols, are the primary contributors to the characteristic astringency of tea infusions[10,38,39]. The overall sensory quality, however, is determined by the balance of metabolites; an optimal ratio of catechins to amino acids (especially theanine) is crucial for achieving a harmonious flavor profile that combines mellowness with umami.
Catechins metabolism and its molecular regulation: key processes, metabolic enzymes, and regulators
-
Catechins are flavonoids biosynthesized via the phenylpropanoid pathway. They are categorized into non-galloylated catechins (e.g., epicatechin) and galloylated catechins (e.g., epigallocatechin gallate, EGCG) based on the presence of a galloyl moiety[40−42]. The genes encoding these key enzymes have been identified[43−45] (Fig. 4a).
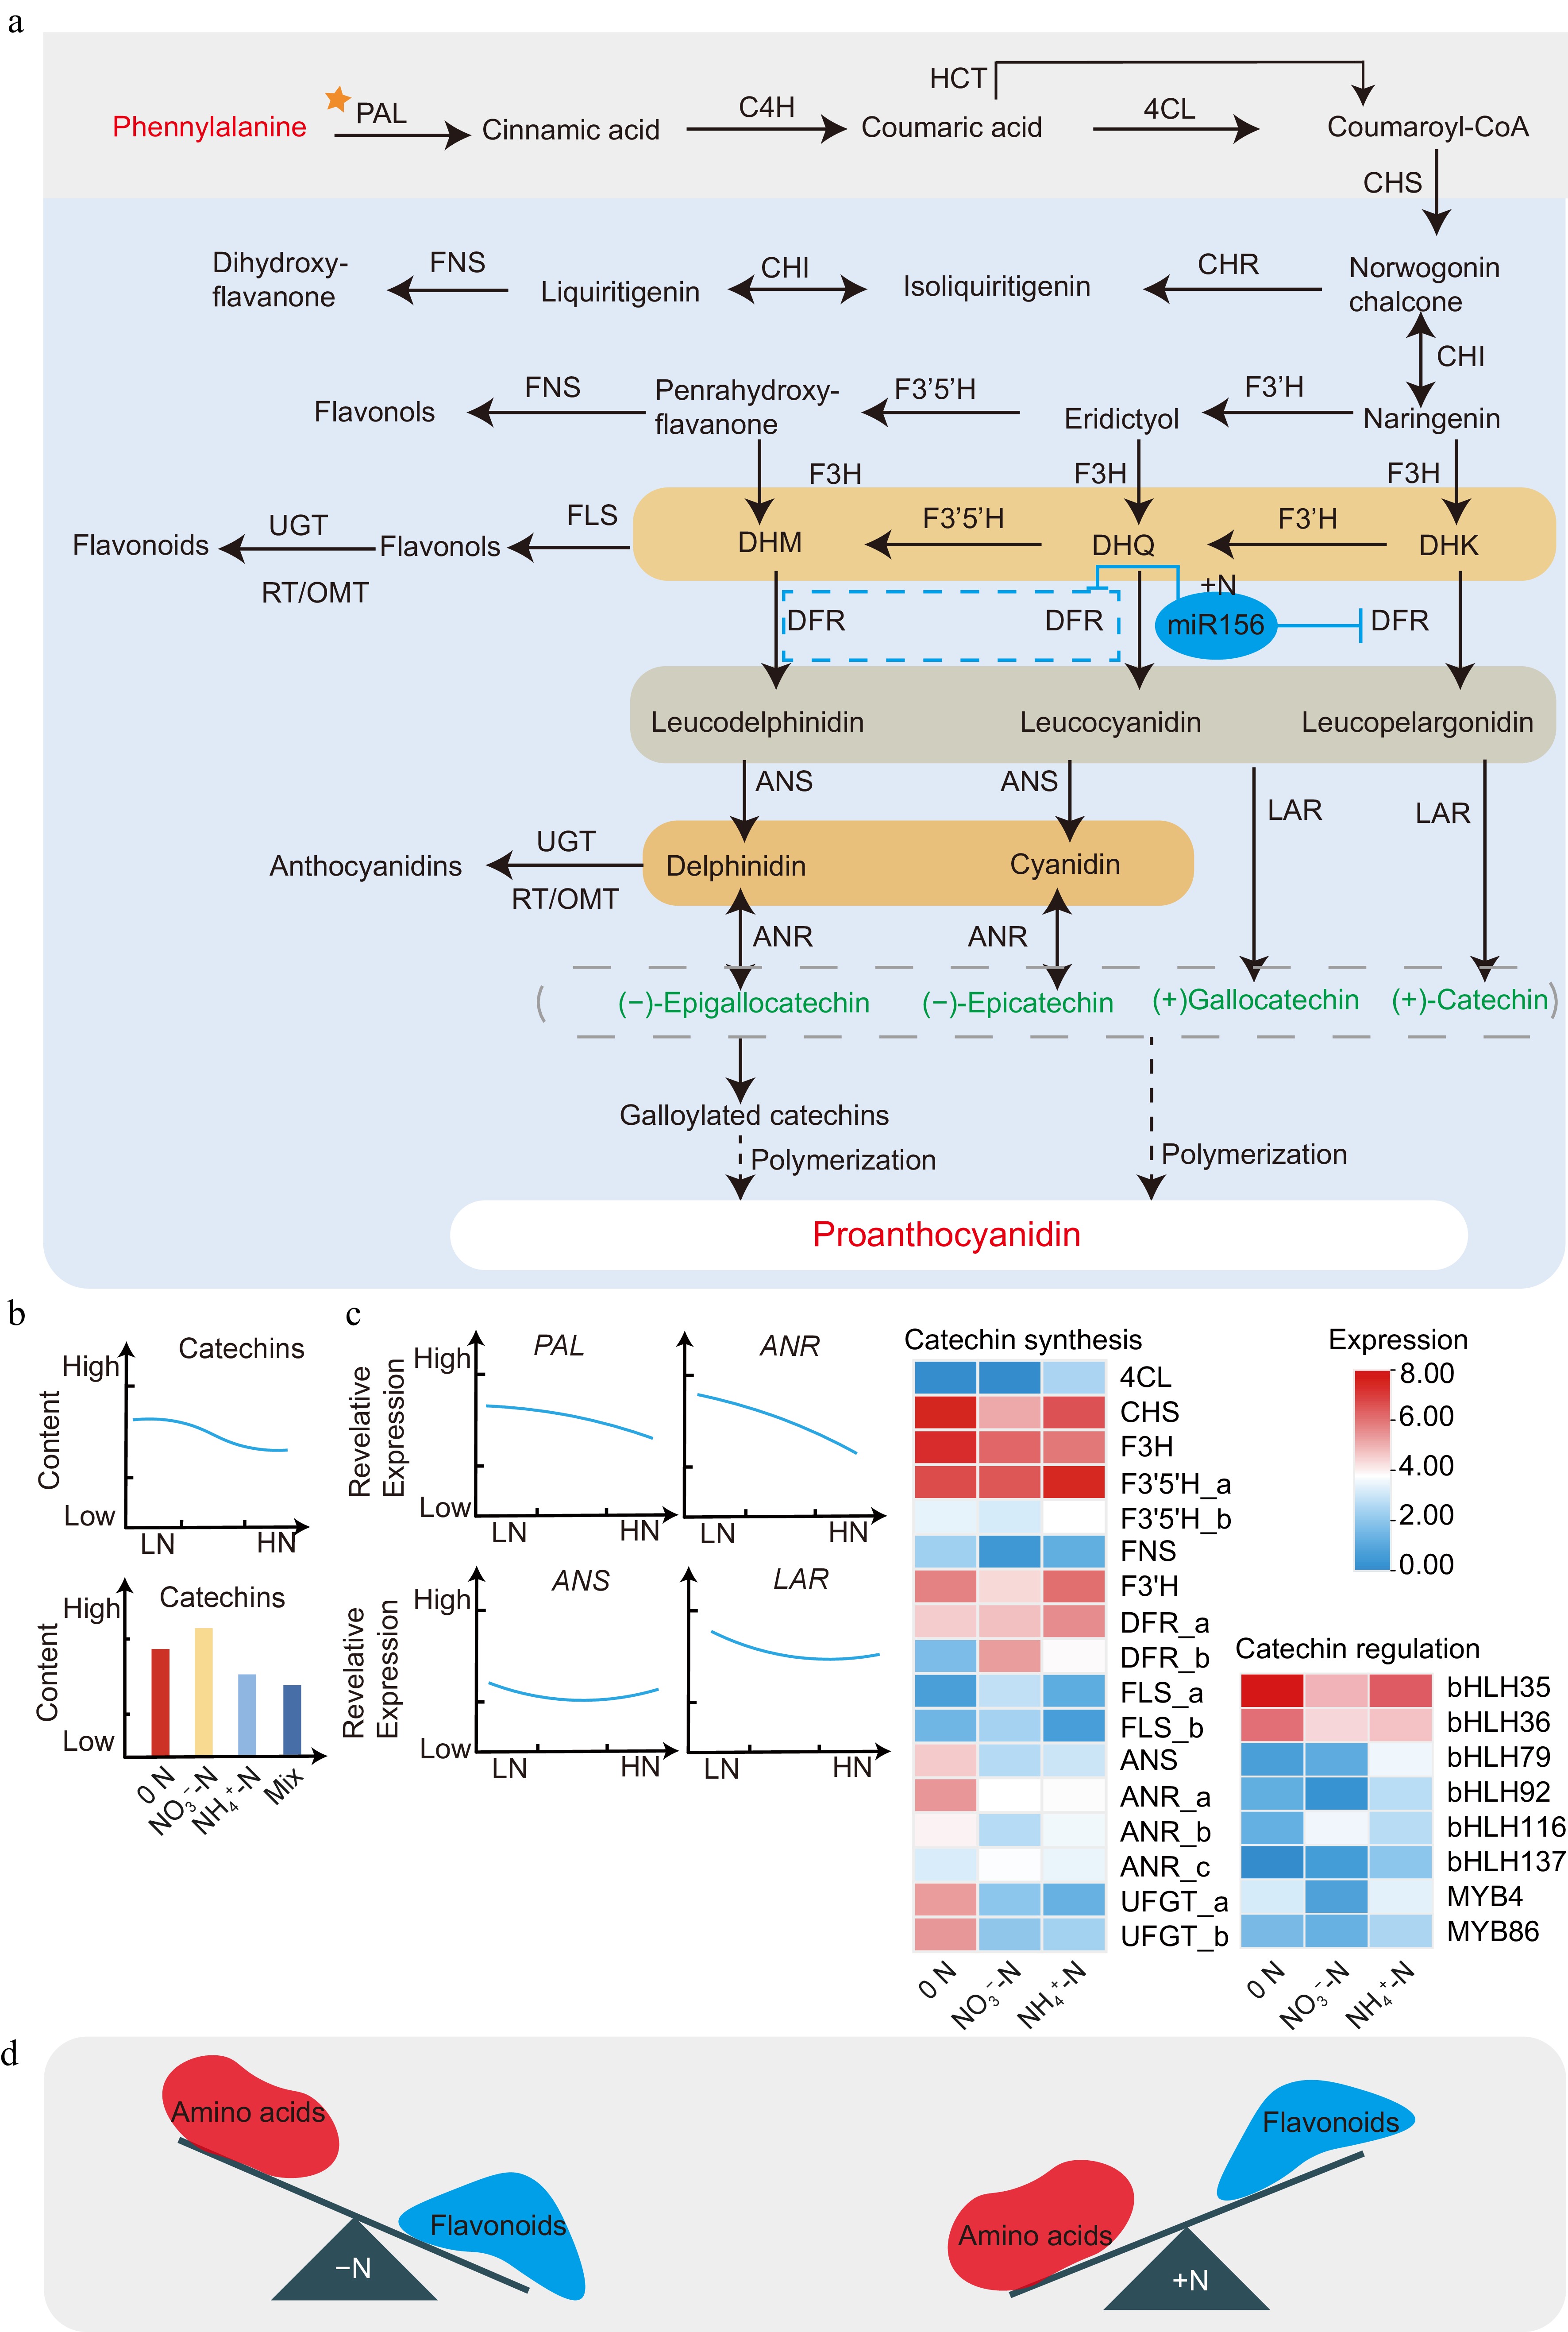
Figure 4.
N regulates catechins biosynthesis and accumulation in tea shoots. The deficiency of N and the presence of NO3−−N stimulate the biosynthesis and accumulation of catechins. Flavonoids and amino acids accumulate antagonistically in tea plants: low N promotes the accumulation of flavonoids and inhibits the accumulation of amino acids; high N promotes the accumulation of amino acids and inhibits the accumulation of flavonoids. (a) Catechins biosynthetic pathway; (b) catechins content under different N levels and forms; (c) relative expression under different N levels and forms; (d) N regulates flavonoids and amino acid accumulation[32,40,46−48]. Abbreviations: Phenylalanine ammonia lyase (PAL), Cinnamic acid 4-hydroxylase (C4H), 4-coumarate: CoA ligase (4CL), Chalcone synthase (CHS), Chalcone reductase (CHR), Chalcone isomerase (CHI), Flavone synthase (FNS), Flavonoid 8-hydroxylase (F8H), Flavanone 4-reductase (FNR), Flavanone 3-hydroxylase (F3H), Flavanone 3’-hydroxylase (F3’H), Flavanone 3’,5’-hydroxylase (F3’5’H), Dihydrokaempferol (DHK), Dihydroquercetin (DHQ), Dihydromyricetin (DHM), Flavonol synthase (FLS), Dihydroflavonol 4-reductase (DFR), Anthocyanidin synthase (ANS), UDP-glucose flavonoid 3-O-glucosyltransferase (UFGT), O-methyl transferases (OMT), Leucoanthocyanidin reductase (LAR), Anthocyanidin reductase (ANR). HN, high N level; LN, low N level; NN, normal N level.
The catechin biosynthetic pathway is tightly regulated at multiple levels. Transcription factors (TFs) from the MYB family, such as CsMYB5 and CsMYB75, directly bind to the promoters of key structural genes like CsLAR and CsANR[49,50]. These MYB TFs often form the MYB-bHLH-WD40 (MBW) complex with partners like bHLH (e.g., TT8) and WD40 (e.g., TTG1) to activate the pathway[51]. Other TFs, including CsTCP3, CsTCP4, and CsTCP14, fine-tune this regulation either independently or in concert with the MBW complex. Beyond transcriptional control, post-transcriptional and post-translational mechanisms are crucial[52]. For instance, the CsbZIP1-CsmiR858a-CsMYBL2 module integrates environmental signals like UV-B or cold to regulate anthocyanin and catechin biosynthesis[53]. Dynamic DNA methylation across seasons and phosphorylation of CsWD40 by CsMPK4a under drought stress further illustrates the sophisticated multi-layered regulation of catechin metabolism[54,55].
Metabolism and accumulation of catechins in response to N status
-
N availability exerts a profound influence on catechin accumulation, typically exhibiting an inverse relationship. Low-N conditions consistently promote catechin biosynthesis and accumulation[32,47,48,56,57] (Fig. 4b). This is mediated by the upregulation of key structural genes, including CsPAL, CsCHS, CsF3H, CsDFR, CsANS, CsLAR, and CsANR. Concurrently, the expression of regulatory components, such as members of the MBW complex (e.g., bHLH35, bHLH36), is also enhanced under N limitation. Conversely, high N levels suppress the pathway, potentially through mechanisms involving CsmiR156-mediated repression of CsSPL and CsDFR.
The form of N also plays a critical role. Compared to NO3−, NH4+ nutrition tends to upregulate specific TFs like MYB4, MYB86, bHLH79, bHLH92 and bHLH137, indicating distinct signaling pathways for different N forms[47] (Fig. 4c). This N-mediated regulation is adaptable; under biotic stress, a strategic reduction in N application can simultaneously enhance plant resistance and stimulate defense-related catechin biosynthesis.
While transcriptional regulation is well-documented, post-translational modifications (PTMs) represent a frontier in understanding N regulation. Our previous work revealed that ubiquitination modifies key enzymes like ANS and ANR under N deficiency[15]. This finding underscores that N regulates catechin metabolism at multiple levels. Future research should prioritize the identification of specific E3 ubiquitin ligases and kinases that target the catechin metabolic machinery, and elucidate how these PTMs are modulated by N signaling.
N regulates the quality characteristics of tea given by catechins
-
By governing catechin accumulation in the harvested shoots, N management directly shapes the processing aptitude and final quality of manufactured tea. The elevated catechin levels under low N or NO3−-dominant nutrition (Fig. 4b) have divergent implications for different tea types[14,19−21,32,46,58].
For unfermented teas like green tea, excessive catechins can lead to undesirable astringency. Therefore, a fertilization strategy that ensures moderate N supply (often with a preference for NH4+) is recommended to maintain a balanced catechin-to-theanine ratio, favoring umami and reducing harshness[59].
In contrast, for fermented teas (black, dark, oolong tea), a higher initial catechin content is advantageous. During the processing of black tea, catechins are oxidized and polymerized into theaflavins and thearubigins, collectively known as tea pigments. This transformation reduces astringency and imparts the characteristic bright red color and brisk flavor to the infusion[60−62]. Consequently, for tea destined for fermented products, a strategic reduction in N fertilizer can be employed to elevate catechin levels in fresh shoots, thereby guaranteeing the formation of distinct quality characteristics post-processing. This practice allows growers to tailor fertilization strategies to the target market and tea product, aligning agronomic inputs with desired quality outcomes.
-
Caffeine, the most abundant purine alkaloid in tea, confers a characteristic bitter taste and exerts a stimulating effect on the central nervous system[63]. It accumulates predominantly in new shoots, which contain approximately 3%–5% caffeine by dry weight, alongside other alkaloids such as theobromine and theophylline[10].
The primary caffeine biosynthesis pathway proceeds through a series of methylation steps: xanthosine → 7-methylxanthosine → 7-methylxanthine → theobromine → caffeine. The key enzyme, tea caffeine synthase (TCS), catalyzes the final two N-methylation steps[64,65]. This pathway is transcriptionally regulated; for instance, the transcription factor CsMYB18 directly activates CsTCS1 expression to promote caffeine production. Following synthesis, intracellular transport of caffeine is facilitated by purine permeases (PUPs). Notably, the expression of CsPUP1, CsPUP3.1, and CsPUP10.1 shows a significant negative correlation with leaf caffeine content, suggesting their potential role in caffeine compartmentalization or remobilization[66]. Catabolism initiates via N-demethylation catalyzed by N-demethylases (NDMs), followed by the action of xanthine dehydrogenase (XDH). A recent study demonstrated that CsXDH1 expression is induced by continuous strong light, promoting caffeine degradation in leaves[67].
While the core metabolic pathway is established, the regulatory mechanisms linking caffeine metabolism to N nutrition remain comparatively less explored. A key insight emerges from distinguishing between short-term and long-term N fertilization effects. In short-term studies, both N forms, and levels, exert a significant influence. NH4+ is more effective than NO3− in promoting caffeine accumulation in new shoots[68,69]. Similarly, higher short-term N application consistently elevates caffeine content, a response strongly associated with the upregulation of CsTCS1 gene expression[14,17,19,70,71].
However, this effect appears adaptable over the long term. Under field conditions, long-term application of high N doses does not necessarily lead to a sustained increase in leaf caffeine content[32]. This discrepancy between short-term responsiveness and long-term stability suggests the presence of compensatory homeostatic mechanisms, possibly involving increased catabolism or altered partitioning, which are activated under chronic high-N supply to maintain metabolic balance.
This nuanced understanding is critical for quality-oriented management. The bitter taste contributed by caffeine must be balanced against other flavor components. The transient increase in caffeine following short-term N application might be leveraged in specific management practices, whereas the long-term stability indicates that caffeine content is not indefinitely scalable through N fertilization alone. Future research should prioritize elucidating the N-sensing pathways that regulate CsTCS1, and the potential role of catabolic genes in mediating the long-term acclimation of caffeine metabolism to N status.
-
Aroma is a paramount quality attribute that defines the character and market value of tea. Over 600 volatile organic compounds (VOCs) have been identified in tea, which can be grouped into three primary categories based on their aroma characteristics: (1) unsaturated aliphatic derivatives (e.g., cyanoalcohols, cyanoaldehydes) impart fresh and grassy notes; (2) aromatics and their derivatives (e.g., benzyl alcohol, phenylethanol, phenylacetaldehyde, methyl salicylate) contribute floral and fruity scents; and (3) terpene derivatives (e.g., geraniol, linalool, nerolidol) also provide floral and fruity aromas[3]. The specific aromatic profile of a tea is determined by the unique composition and abundance of these VOCs.
Six tea types exhibited distinct aromas. Green tea mainly displays fresh, chestnut, and floral aromas[72]. Black tea is typically known for its sweet, floral, and fruity aroma. In particular, Keemun black tea stands out for its distinctive 'Keemun aroma', which is primarily attributed to terpene alcohols[73]. White tea shows pekoe and floral aromas as its main characteristics, with aldehydes being the primary contributing compounds[74]. Large-leaf yellow tea is a unique, lightly fermented tea that emits an aroma similar to fried rice and a roasted flavor; pyrazines play a crucial role in presenting this aroma[75]. Oolong tea is mainly a floral and roasted aroma, and parylene and pyrrole are the main flavor-presenting substances of the roasted aroma[76]. The most significant aroma of dark tea is the aged aroma, and methoxybenzene compounds produced during the fermentation process are the primary contributors[77].
N regulates the accumulation of volatile organic compounds in tea plant leaves
-
The formation of a high-quality tea aroma begins with the optimal biochemical composition of the fresh leaves. N nutrition plays a critical role in this process, regulating not only taste-related metabolites, but also the VOCs.
Optimal N application enhances desirable floral and fruity aromas. It upregulates gene encoding enzymes like β-glucosidase and β-sakuranosidase, leading to increased levels of β-linalool and linalool oxides (Fig. 5a). Furthermore, compounds such as methyl salicylate, nerolidol, and nerolidol tertiary alcohol, which contribute these pleasant odors, are newly synthesized or enhanced under balanced N supply[79]. This demonstrates that proper N management can actively promote the formation of positive aroma attributes.
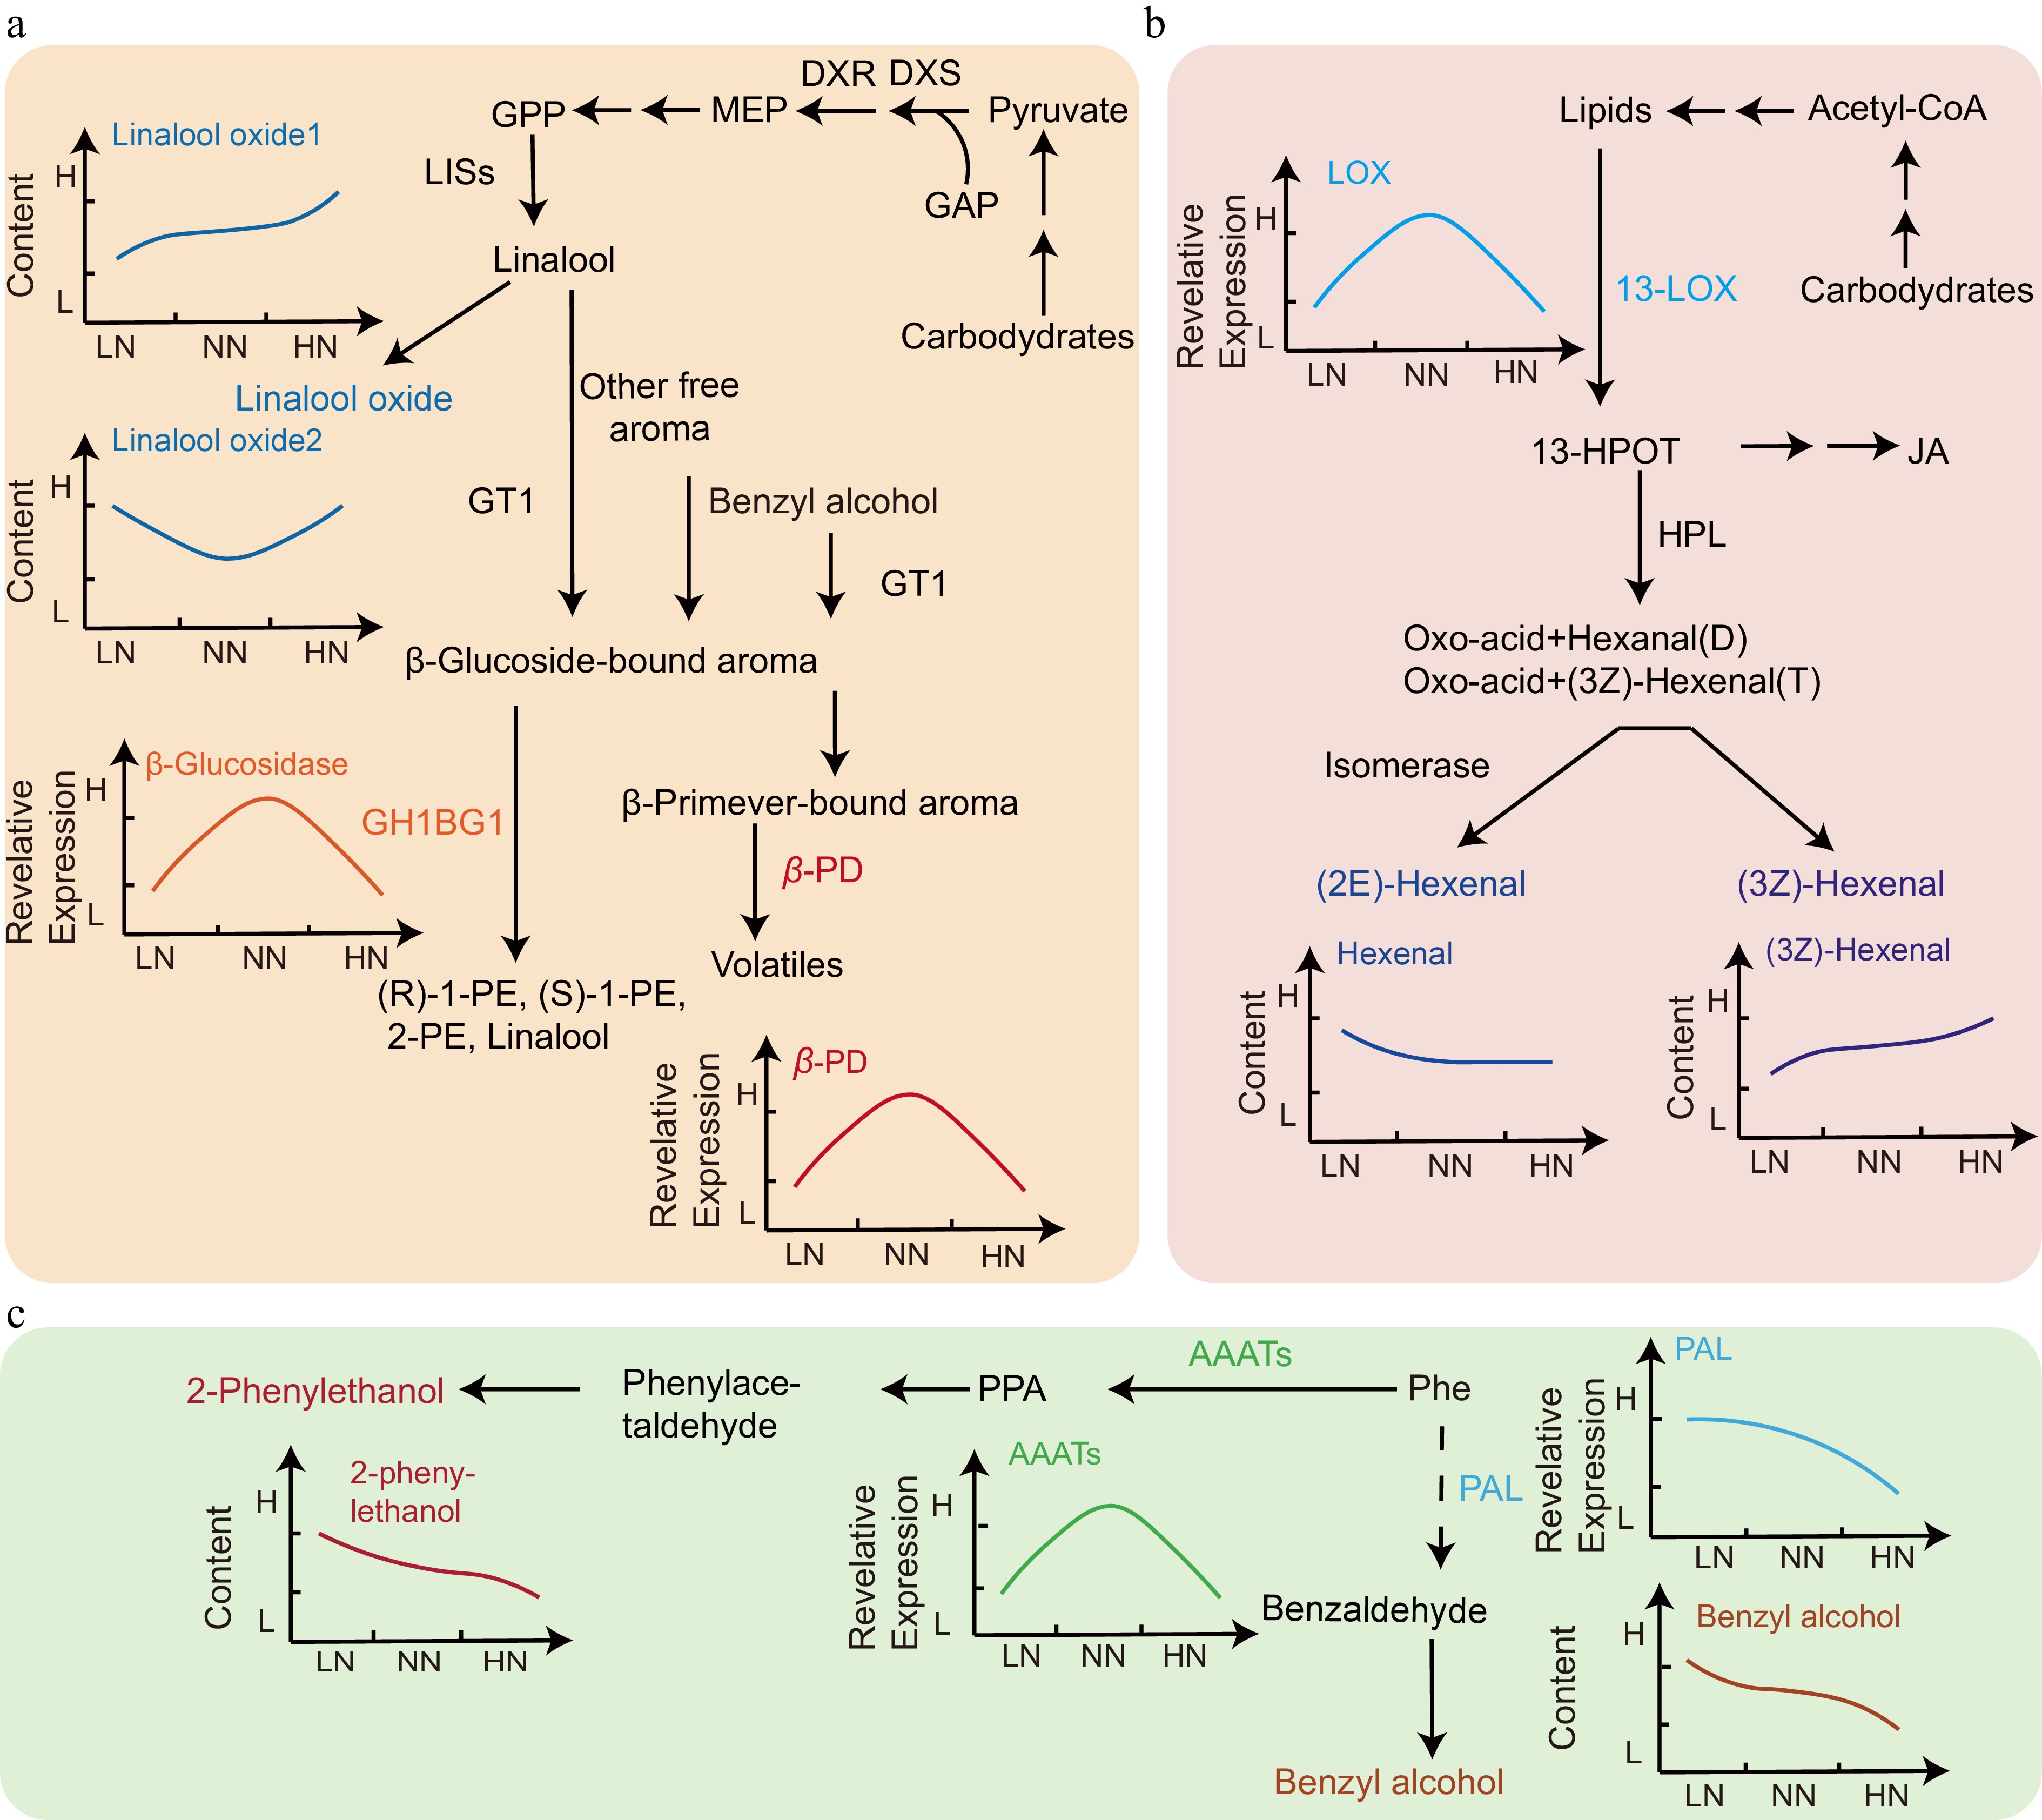
Figure 5.
N regulates the biosynthesis and accumulation of VOCs in tea plants and their effects on tea aroma. N deficiency or excessive N inhibits the accumulation of tea aroma compounds. (a) MEP pathway; (b) LOX pathway; (c) L-Phe pathway; (d) N forms and levels regulate VOCs accumulation in tea plants and their effects on tea aroma. In (d), the up and down arrows represent increases and decreases in aroma compound contents, respectively[32,78−80]. Abbreviations: GPP, geranyl diphosphate; LISs, linalool synthases; GT, glycosyltransferase; β-PD, β-Primeverosidase; PE, phenylethanol; LOX, lipoxygenase; HPL, hydroperoxide lyase; AAATs, aromatic amino acid aminotransferases; PPA, phenylpyruvic acid. HN, high N level; LN, low N level; NN, normal N level.
Conversely, N deficiency has detrimental effects. It hinders the biosynthesis of VOCs overall. For example, N deficiency significantly downregulates the expression of CsLOX, a key gene encoding lipoxygenase in the lipid-derived volatile pathway[80] (Fig. 5b).
Excessive N application is equally detrimental, as it increases the fatty acid content in leaves, which can be converted into VOCs that impart an undesirable grassy flavor[78]. Simultaneously, high N levels downregulate genes in the phenylalanine biosynthesis pathway, reducing the production of floral compounds like phenylmethanol and 2-phenylethanol[32] (Fig. 5c). This highlights a trade-off, where over-fertilization can suppress key aromatic pathways.
Finally, the interaction between N with other nutrients is crucial; for instance, reducing P fertilization can enhance the distinctive 'regional aroma' of Wuyi Rock Tea[81], and K application promotes the synthesis of floral terpenoids[82]. Future research should explore these interactions across different tea types and investigate the combined effects of N with other elements on the final aroma profile.
-
N availability acts as a central switch that reprograms the metabolic network in tea plants, dynamically altering the synergistic and antagonistic relationships among key quality-related compounds. Understanding this crosstalk is crucial for predicting how N management shapes the final, integrated quality of tea.
A fundamental trade-off regulated by N is the antagonism between N-rich and carbon-rich metabolites. High N application promotes the synthesis of amino acids but often at the expense of flavonoids like catechins (Fig. 4d). This inverse relationship stems from the competition for shared carbon skeletons and energy. Notably, the form of N storage within the plant can shift under excessive supply. Although theanine is the main N storage source under moderate conditions, high N levels lead to a significant increase in the ratio of arginine to total amino acids (Fig. 2a). This suggests that arginine may become the preferred N storage form under extreme N consumption[17]. This shift has direct implications for NUE and quality.
The coordination between other metabolite pairs is also modulated by N status. Under short-term N fertilization, caffeine and catechins often show positively correlated accumulation trends[67,68]. This synergy may reflect a shared activation of secondary metabolic pathways under specific N signaling. Conversely, N levels critically influence the balance between desirable and undesirable aroma profiles. Low N conditions tend to promote the accumulation of floral-scented compounds (e.g., benzyl alcohol, linalool oxides) while suppressing grassy-scented lipids. This favorable profile is often reversed under high N, which stimulates the production of green, grassy volatile compounds, creating an aroma quality antagonism[32,78,83] (Fig. 5).
In summary, N does not merely regulate individual metabolite pathways in isolation. It functions as a master integrator of primary and secondary metabolism, determining the allocation of resources and thereby establishing the final balance of taste and aroma compounds. Deciphering this crosstalk is therefore essential for developing precision fertilization strategies that move beyond maximizing single components, and instead aim to optimize the synergistic and sensory-balanced metabolite profile that defines premium tea quality.
-
The synthesis presented in this review establishes that N functions as a central signaling molecule, orchestrating a complex metabolic network that determines the final quality of tea. Moving forward, the key challenge lies in translating this mechanistic understanding into practical strategies that reconcile high quality with environmental sustainability and economic viability. This necessitates a paradigm shift from yield-centric fertilization to precision nutrient management guided by plant metabolism. Future efforts should converge on the following interconnected fronts.
Precise fertilization ensures that the supply of nutrients match the quality targets
-
Current fertilization in tea plantations often exceeds agronomic demand, with average inputs in China reaching 796 kg N + P2O5 + K2O ha−1 yr−1, leading to nutrient imbalances and quality decline in approximately 30% of cases[82,84−87]. The established inverse relationship between N availability and the biosynthesis of carbon-intensive metabolites (e.g., catechins) vs N-rich compounds (e.g., theanine) provides a scientific basis for quality-oriented fertilization.
Future strategies must be product-specific. For instance, the production of high-umami green tea would benefit from moderate ammonium-N supply to enhance theanine while curbing excessive catechins[88]. Conversely, for black tea requiring abundant catechin substrates for oxidation, a controlled, slightly reduced N supply could be optimal. Implementing this requires dynamic nutrient management informed by soil tests, leaf spectral diagnosis, and clear metabolic quality benchmarks, moving beyond uniform annual applications[80,89,90].
Synergistic nutrient management for enhanced efficiency and quality
-
N does not act in isolation. Its effect on quality metabolites is modulated by interactions with other nutrients, as evidenced by the roles of P, K, and Mg in theanine transport and terpenoid synthesis, respectively[28−31,82]. Therefore, balanced fertilization is critical.
Future research should focus on establishing integrated nutrient formulae that optimize the synergy between N, P, K, Mg, and other elements for targeted tea types. Furthermore, the development and adoption of enhanced-efficiency fertilizers, such as controlled-release, organic with inorganic or stabilized N forms, can synchronize nutrient release with plant demand, thereby improving NUE and minimizing environmental leakage[91−94].
Harnessing the rhizosphere microbiome for nutrient efficiency
-
The soil microbiome is a crucial, yet underexplored, mediator of N cycling and plant nutrition. Agronomic practices, including fertilization, alter microbial community structure, which in turn influences nutrient availability and plant physiology. Emerging evidence suggests that specific root-associated microbiota can regulate N homeostasis and enhance theanine synthesis[95]. Intercropping systems, which modify the soil microbiome, have also been linked to improved quality[96−98].
This opens a promising frontier for microbial-based interventions. Future work should aim to identify and formulate consortia of beneficial microbes that can act as bio-fertilizers or bio-stimulants. These microbial tools could enhance N uptake, influence the expression of plant metabolic genes, and ultimately elevate quality under reduced chemical N input, contributing to a more sustainable production system.
Towards smart cultivation: data-driven and intelligent management
-
The complexity of soil-plant-environment interactions calls for advanced management tools. The integration of smart agriculture technologies—including Internet of Things sensors for real-time soil and plant monitoring, drone-based hyperspectral imaging, and AI-powered data analytics can enable true precision farming[89,90,99].
The development of decision-support systems that integrate real-time field data, weather forecasts, and mechanistic models of nutrient-metabolite relationships will be transformative. Such platforms could provide growers with actionable insights to dynamically adjust fertilization, not just for yield, but to steer the crop towards a predefined quality profile, ensuring both resource efficiency and product consistency.
Genetic improvement: breeding for the next generation of tea cultivars
-
The improvement of NUE in tea plants can be achieved not only through enhanced fertilization practices but also by selecting and breeding high NUE varieties. Extensive research has been conducted on high NUE genes in major crops, such as rice and maize, focusing on optimizing root systems, nutrient assimilation and transport activities, and resistance[100]. However, studies focusing on tea plants have been limited because of various constraints. Nevertheless, multi-omics joint analysis and molecular biology techniques can be employed to identify functional genes so that they can be used for future design breeding. We aimed to shorten the breeding cycle of high-quality tea plant varieties, enhance efficiency, and reduce costs. When stable gene transformation can be performed in tea plants, we anticipate initiating a sustainable Green Revolution for this crop.
-
Achieving sustainable premium tea production requires a concerted transition from empirical practices to a science-based framework. By integrating precision nutrient management, microbial biotechnology, smart farming technologies, and advanced genetics, the tea industry can proactively design cultivation systems that optimize the intricate metabolic network governed by nitrogen. This integrated approach promises to secure the future of tea production, ensuring exceptional quality, environmental stewardship, and economic resilience.
-
The authors confirm their contributions to the paper as follows: Yan X: conceptualization, writing–original draft, visualization, writing−review and editing. Lin S: conceptualization, visualization, writing–review and editing. Zhang Z and Ruan J: conceptualization, writing–review and editing, supervision, funding acquisition. Wang J, Yang T, and Liu M: writing–review and editing. All authors reviewed the results and approved the final version of the manuscript.
-
Data sharing is not applicable to this article as no datasets were generated or analyzed during the current study.
-
The authors declare that they have no conflict of interest.
-
# Authors contributed equally: Xuehang Yan, Shijia Lin
- Copyright: © 2026 by the author(s). Published by Maximum Academic Press, Fayetteville, GA. This article is an open access article distributed under Creative Commons Attribution License (CC BY 4.0), visit https://creativecommons.org/licenses/by/4.0/.
-
About this article
Cite this article
Yan X, Lin S, Wang J, Yang T, Liu M, et al. 2026. Nitrogen regulates the biosynthesis of key secondary metabolites in tea plant (Camellia sinensis): a review. Beverage Plant Research 6: e034 doi: 10.48130/bpr-0026-0012 

Nitrogen regulates the biosynthesis of key secondary metabolites in tea plant (Camellia sinensis): a review
- Received: 26 January 2026
- Revised: 28 February 2026
- Accepted: 09 March 2026
- Published online: 08 September 2026
Abstract: Nitrogen (N) plays a dual role in tea plants, serving as both an essential nutrient for growth, and a key regulator of quality-related secondary metabolism. Recent research has concentrated on elucidating how different levels or forms of N influence key secondary metabolites, such as amino acids, flavonoids, caffeine, and aroma compounds, and how these metabolites collectively determine the flavor of tea. However, excessive N application can adversely affect tea quality and reduce nitrogen use efficiency (NUE). This review systematically examines recent advances in understanding how N signaling modulates these pathways, with particular emphasis on the molecular mechanisms underlying N-regulated gene expression, enzyme activity, and inter-pathway crosstalk. We further discuss how this knowledge informs the development of targeted agronomic practices and breeding strategies aimed at achieving sustainable tea production—optimizing quality while enhancing NUE under reduced N input.
-
Key words:
- Nitrogen /
- Quality /
- Biosynthesis /
- Transport /
- Regulates /
- Camellia sinensis