











-
Birds in ecological communities are continuously facing dynamic predation pressures and have to accurately assess diverse predator characteristics[1,2]. Predation pressure is a key selective force in the evolution of adaptive behavioral strategies in birds. By exerting a powerful influence on avian communities, predators drive the development of effective anti-predator responses among prey species[3−5]. Thus, prey species enhance the efficacy of collective defense, which contributes to the formation and stability of the avian community. Mobbing behavior represents a widespread anti-predator strategy in birds to mitigate predation risk. This active defense mechanism involves the aggregation of individuals to assemble and attack predators, thereby reducing the immediate threat or predation pressure[6,7].
Although mobbing is universal in avian communities, there is significant controversy about drivers of avian mobbing assemblage formation. The decision of birds to participate in a mobbing assemblage and the intensity of their involvement are influenced not only by predators but also by a multitude of factors[8,9], including avian body size, age, foraging stratum, interspecific sociality, seasonal variations, and the composition of the local avian community[10,11]. Substantial evidence indicates that participation in mobbing events is predominantly observed among small-bodied bird species[12,13]. The frequency and intensity of mobbing behavior increase during the breeding season[9,14]. The influx of winter migrants can alter local avian community composition and lead to a greater diversity of species participating in mobbing[15]. Apart from biological factors, environmental conditions such as habitat structure and temperature also play a crucial role in shaping mobbing behavior. Complex understory vegetation promotes more intense mobbing behavior[16], whereas elevated ambient temperatures reduce mobbing motivation in the Great Tit (Parus major)[17].
The Collared Owlet (Taenioptynx brodiei) is a common diurnal raptor with a wide distribution in Eastern Asia and Southern Asia; thus, it should be an ideal predator to explore the diversity of mobbing behavior of bird assemblages. As a resident small strigiform raptor in the Hengduan Mountains forest ecosystem, the Collared Owlet occupies a predator position in the food chain. Its diet encompasses passerines and other small to medium-sized birds, thereby exerting sustained natural selection pressure on the local avian community[12,18]. Compared to migratory raptors, its sedentary nature makes it an important driver for long-term adaptation by bird assemblages. They produce highly repetitive calls with distinct frequency bands. These acoustic features enhance signal transmission in forest environments, allowing the calls to be readily distinguishable from background noise. This makes the Collared Owlet an ideal model system for investigating predator–prey interactions in the study region.
In this study, we conducted 113 playback trials of Collared Owlet vocalizations in Mt. Gongga, China, to: (1) identify differences in avian community and mobbing behavior across seasons and elevational gradients; and (2) ascertain the effects of phylogenetic relationships, functional traits, and environmental factors on bird mobbing behavior. These objectives have implications for further elucidating the anti-predator strategies of birds and for enriching our understanding of the formation patterns and mechanisms of bird mobbing behavior.
Based on the ecological framework outlined above, we propose the following hypotheses and predictions. First, we hypothesize that avian mobbing responses will be stronger in seasons and habitats associated with higher energetic demands and increased predation risk, particularly during the breeding season and at elevations where predator exposure is more frequent. Second, we predict that mixed-species flocks, especially those dominated by small-bodied and high-maneuverability species, will exhibit higher mobbing participation and intensity due to enhanced collective vigilance and reduced individual risk. Third, we expect that resident species will show stronger and more consistent mobbing responses compared to migratory species, reflecting differences in local experience with predator cues.
-
This research implemented three survey transects within each of the two distinct elevational ranges (1,800–2,200 m, where the Collared Owlet is common, and 2,800–3,200 m, where the species has not been historically recorded), resulting in a total of six transects on eastern Mt. Gongga in Hailuogou (29°30′–29°40′ N, 101°50′–102°10′ E). Playback experiments were executed along 4 km transects at two elevations (Fig. 1). Primary forest is located at 2,800–3,200 m, and secondary forest is located at 1,800–2,200 m with a diverse bird community[19]. Each transect was surveyed at least once in both morning and afternoon periods, with playback trials on the same transect separated by more than 24 h. A minimum interval of 30 min was maintained between consecutive playback trials, and at locations spaced more than 400 m apart. The playback experiments were conducted from March to August 2024 (breeding season) and September to November 2024 (non-breeding season), with daily trials occurring between 07:00–11:00 and 14:00–18:00. This schedule was designed to avoid the snow-covered period (December to February), when low temperatures and reduced avian activity and abundance occur. A total of four surveys were carried out during the breeding season and two during the non-breeding season, with each survey lasting 15 to 20 d.
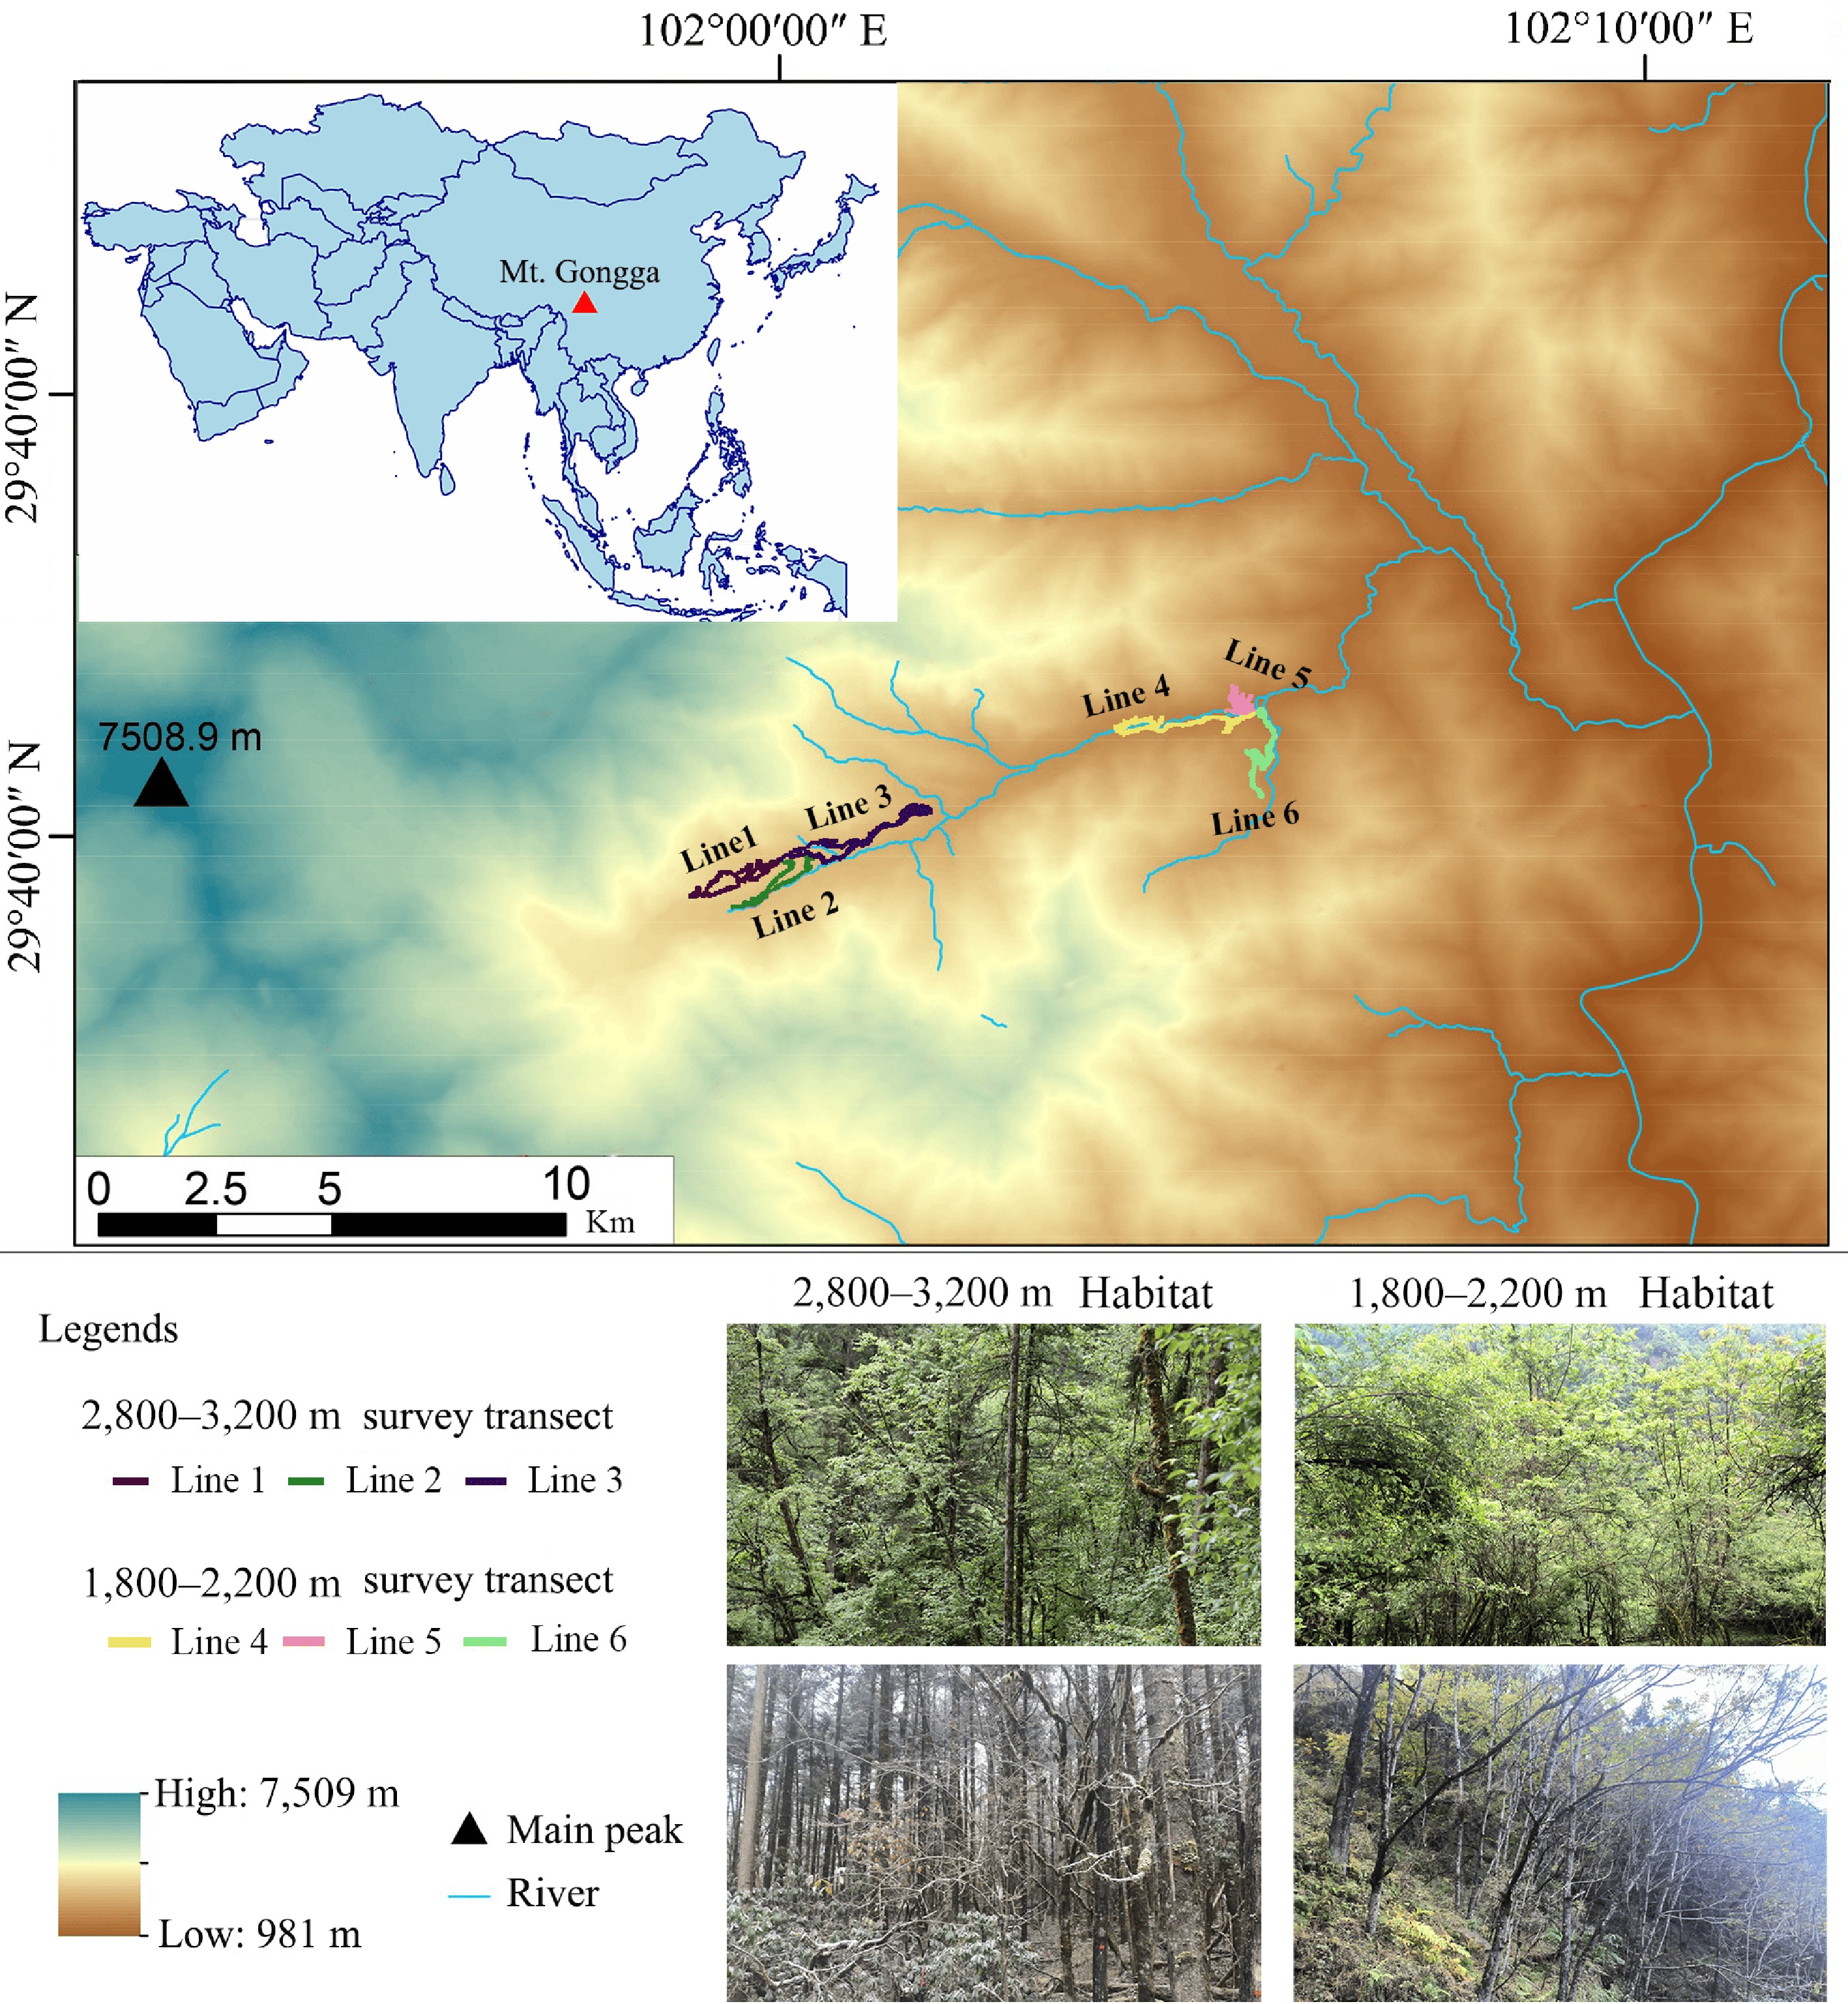
Figure 1.
Study area and survey transect. The base map of China was obtained from Natural Earth (
www.naturalearthdata.com/ ), and visualized in R.Playback protocol and scoring of recordings
-
Playback experiments were conducted shortly after visually or acoustically detecting active bird flocks within a 30-m radius. This prerequisite ensured that a comparable baseline of avian activity was established at each location prior to the broadcast, thereby minimizing the confounding effects of ambient species availability on the number of responding individuals. To ensure that the observed bird mobbing behavior was triggered solely by acoustic cues, visual stimuli such as specimens or models of the Collared Owlet were deliberately excluded from the playback experiments. The vocalizations of the Collared Owlet were broadcast repeatedly for 10 min using a JBL GO3 portable Bluetooth speaker when bird flocks were encountered. The playback volume was set to 80 dB at a distance of 1 m from the speaker, which closely replicates the natural call amplitude of the Collared Owlet and follows standardized protocols for small raptor playbacks in forest environments[20,21]. The speaker was positioned 5–7 m away from the bird flock and mounted at a height of 1.5–1.8 m above the ground. Two observers with camouflage clothing stood more than 10 m from the playback device to minimize potential disturbance. The vocalization of the Collared Owlet was obtained from the Xeno-Canto database (
https://xeno-canto.org/ ). The specific recording selected for playback experiments was XC892514, with a duration of 30 s, which was recorded in Thailand. Although avian vocalizations can exhibit geographic variation, both the Thai population and the Chinese population of the Collared Owlet belong to the same mainland subspecies (G. b. brodiei). Acoustic analysis indicates that the vocal differences within this subspecies across different regions are not significant[22]. In avian behavioral ecology, using a single stimulus track can potentially introduce the risk of acoustic pseudoreplication[23], where responses might reflect traits of a specific recording rather than the predatory species as a whole. While the highly stereotyped and innate nature of strigiform vocalizations[22] and the need to eliminate confounding background noises from multiple public database files justified our approach for cross-elevational comparisons, future studies should ideally employ multiple distinct stimulus tapes to ensure broader generalizability of collective anti-predator responses. During each transect survey, a control experiment using natural sound playback was conducted, ensuring the absence of anthropogenic disturbance. The natural sounds used for the control experiments at different altitude segments were all recorded within the typical habitats of their corresponding altitude ranges. We employed professional recording equipment (SONY, ICD-PX470) and conducted recordings under weather conditions with no precipitation and wind speeds below Beaufort force 3 to minimize interference from extraneous noise. The audio clips selected for playback were carefully screened to ensure they contained no vocalizations from predators or any other alarm calls. The control trials were interspersed randomly with predator playback trials throughout the entire field season, and they were never conducted simultaneously at the exact same location. All control trials utilized identical audio playback equipment and volume settings for sound presentation.For each playback experiment, data were collected on all bird species within a 25-m radius of the speaker. The following variables were recorded for each species: the number of responding individuals, the duration of time individuals stayed within the cluster (response time), the closest approach distance to the speaker (response distance), the average height of bird activity (response height), and the primary vertical stratum of activity. Concurrently, the behaviors exhibited by birds during the mobbing event were systematically recorded and scored (for detailed aggression scores, see Supplementary Table S1). This scoring system assigned higher values to individuals having more intense and aggressive behaviors. Response duration was defined as the time from the first individual exhibiting a mobbing response to the last individual returning to normal activities or leaving the area. Response distance and height were measured using a SNDWAY model Laser Range Finder. Mobbing assemblage duration was measured from the initiation of mobbing behavior by the first bird until all birds resumed normal activities or left the speaker. Foraging strata were classified into five layers: ground, understory, mid-story, upper-story, and canopy. Environmental variables included playback start time and real-time microclimatic conditions, with temperature and humidity measured using a Jian Da Ren Ke COS-04-X auto-logger to record stabilized values.
Mobbing indices and functional traits
-
During playback trials, an aggression score exceeding two was established as the threshold for confirming a species' engagement in mobbing behavior. Playback trials were deemed to elicit standard mobbing behavior under two conditions: 1) eliciting responses from two or more species; or 2) eliciting responses from three or more individuals of a single species. The research investigated avian mobbing behaviors on two ecological levels: individual species responses (response duration, minimum approach distance, mean response height, aggression score, and primary foraging stratum) and group-level responses (comprising species richness of participants, total number of responders, and duration of mobbing events).
For the bird species involved in mobbing events, six morphological traits were obtained from the Life-history and Ecological Traits Database of Chinese Birds[24]. These traits included body mass (g), body length (mm), bill length (mm), wing length (mm), tail length (mm), and tarsus length (mm). Hand-wing index values were obtained from datasets by Sheard et al.[25] and Tobias et al.[26], with mean values applied in further analyses. Dietary composition of mobbing birds was obtained from the aforementioned Chinese bird trait database. Foraging height preferences were derived from the dataset published by Wilman et al.[27]. The foraging height was quantified by calculating the proportion of time each species spent foraging across different vertical strata. Based on the forest structure characteristics of the study area, reference heights for these strata were assigned as 0, 2.5, 5, 10, and 20 m, respectively[13]. The capacity of bird species to form mobbing assemblages was assessed using sociality metrics. This was characterized at two levels: intraspecific sociality, measured as the frequency of conspecific individuals forming groups, and interspecific sociality, represented by the proportion of participation in mixed-species flocks[12]. Taxonomic nomenclature and classification follow the A Checklist on the Classification and Distribution of the Birds of China (Fourth Edition)[28].
Statistical analyses
-
We used the 'MCMCglmm' package to construct a Bayesian phylogenetic mixed model, which assessed the influence of potential factors on avian mobbing behavior[12,29]. The predictor variables can be grouped into three main categories: species-level functional traits (morphological PC1, foraging behavior PC1, hand-wing index, residency status, foraging height, interspecific sociality, intraspecific sociality, and species abundance), environmental and experimental variables (temperature, humidity, elevation, breeding season, and playback time of day), and random effects structure (phylogenetic relationships among species and experimental identity). We downloaded 5,000 pseudo-posterior distribution trees encompassing all responding bird species from
http://birdtree.org (Hackett All Species: a set of 10,000 trees with 9,993 OTUs each)[30,31]. A Maximum Clade Credibility (MCC) tree was then generated using TreeAnnotator v1.10.3 in the BEAST software package[32]. Blomberg's K was calculated to quantify phylogenetic signal for continuous functional traits (Correlations among continuous variables are shown in Supplementary Fig. S1)[33]. Additional phylogenetic signal analyses were performed using the 'phylo.d' function in the 'caper' package and the 'multiPhylosignal' function in the 'picante' package[34]. Prior to model runs, we assessed variance inflation factors (VIFs) for all predictors using the 'vif' function in the 'caper' package and excluded those with VIF > 2 to mitigate multicollinearity. Continuous predictors were Z-score standardized prior to model fitting. The number of model iterations, burn-in period, and thinning interval were set as 330,000, 30,000, and 300, respectively.Chi-square tests were employed to compare differences in mobbing formation (presence/absence of mobbing assemblages) across breeding seasons and elevational bands. When data did not meet the assumptions of the chi-square test, two-tailed Fisher's exact tests were used instead. For continuous mobbing response variables, outliers were removed prior to analysis. Normality was assessed using the Shapiro–Wilk test, and homoscedasticity (homogeneity of variances) was evaluated with Levene's test. If both assumptions were met or sample sizes exceeded[29], Student's t-tests were applied to examine differences in response metrics between seasons and elevations. If assumptions were violated, Wilcoxon rank-sum tests (Mann–Whitney U tests) were used. For categorical mobbing response variables, chi-square tests were used to assess seasonal and elevational differences. When contingency table assumptions were not met, two-tailed Fisher's exact tests were applied. All analyses were conducted in the R statistical software environment (v4.4.2 R Core Team[35]).
Ethical note
-
All procedures in this experiment were conducted following the National Wildlife Conservation Law (
https://en.npc.gov.cn.cdurl.cn/2022-12/30/c_1085104.htm ) and with permission from the Forestry Department of Ganzi Tibetan Autonomous Prefecture. This study was based entirely on the non-contact observation of natural avian behavior. It involved no capture, marking, or physiological intervention of individual birds, caused no physical alteration or long-term impact to their habitat, and resulted in no identifiable harm or welfare compromise to birds. Therefore, formal ethical approval from the Animal Ethics Committee of the College of Life Sciences at Sichuan University was not sought for this research. The volume, frequency, and duration of the playback stimuli in this experiment were carefully calibrated to ensure that the experimental audio closely approximated the acoustic characteristics of natural vocalizations, while remaining below thresholds that could potentially cause auditory damage or undue stress. This calibration was conducted to achieve the scientific objectives while minimizing any potential impact on the study subjects. Crucially, post-playback monitoring confirmed that all individuals resumed normal activities after playbacks. -
A total of 113 playback trials of Collared Owlet vocalizations were conducted. Among these, 90 trials successfully elicited mobbing assemblages, resulting in a mobbing response rate of 79.65%. During these experiments, 72 bird species from 27 families and four orders were recorded, with Passeriformes dominating both in species richness (24 families, 69 species) and individual participation (913 individuals) (Fig. 2). All 10 species with the highest mobbing frequency (MFall > 16%) belonged to Passeriformes (Supplementary Table S2). Green-backed Tit (Parus monticolus) exhibited the highest mobbing frequency, while Sichuan Leaf Warbler (Phylloscopus forresti) mobilized the largest number of individuals (Table 1).
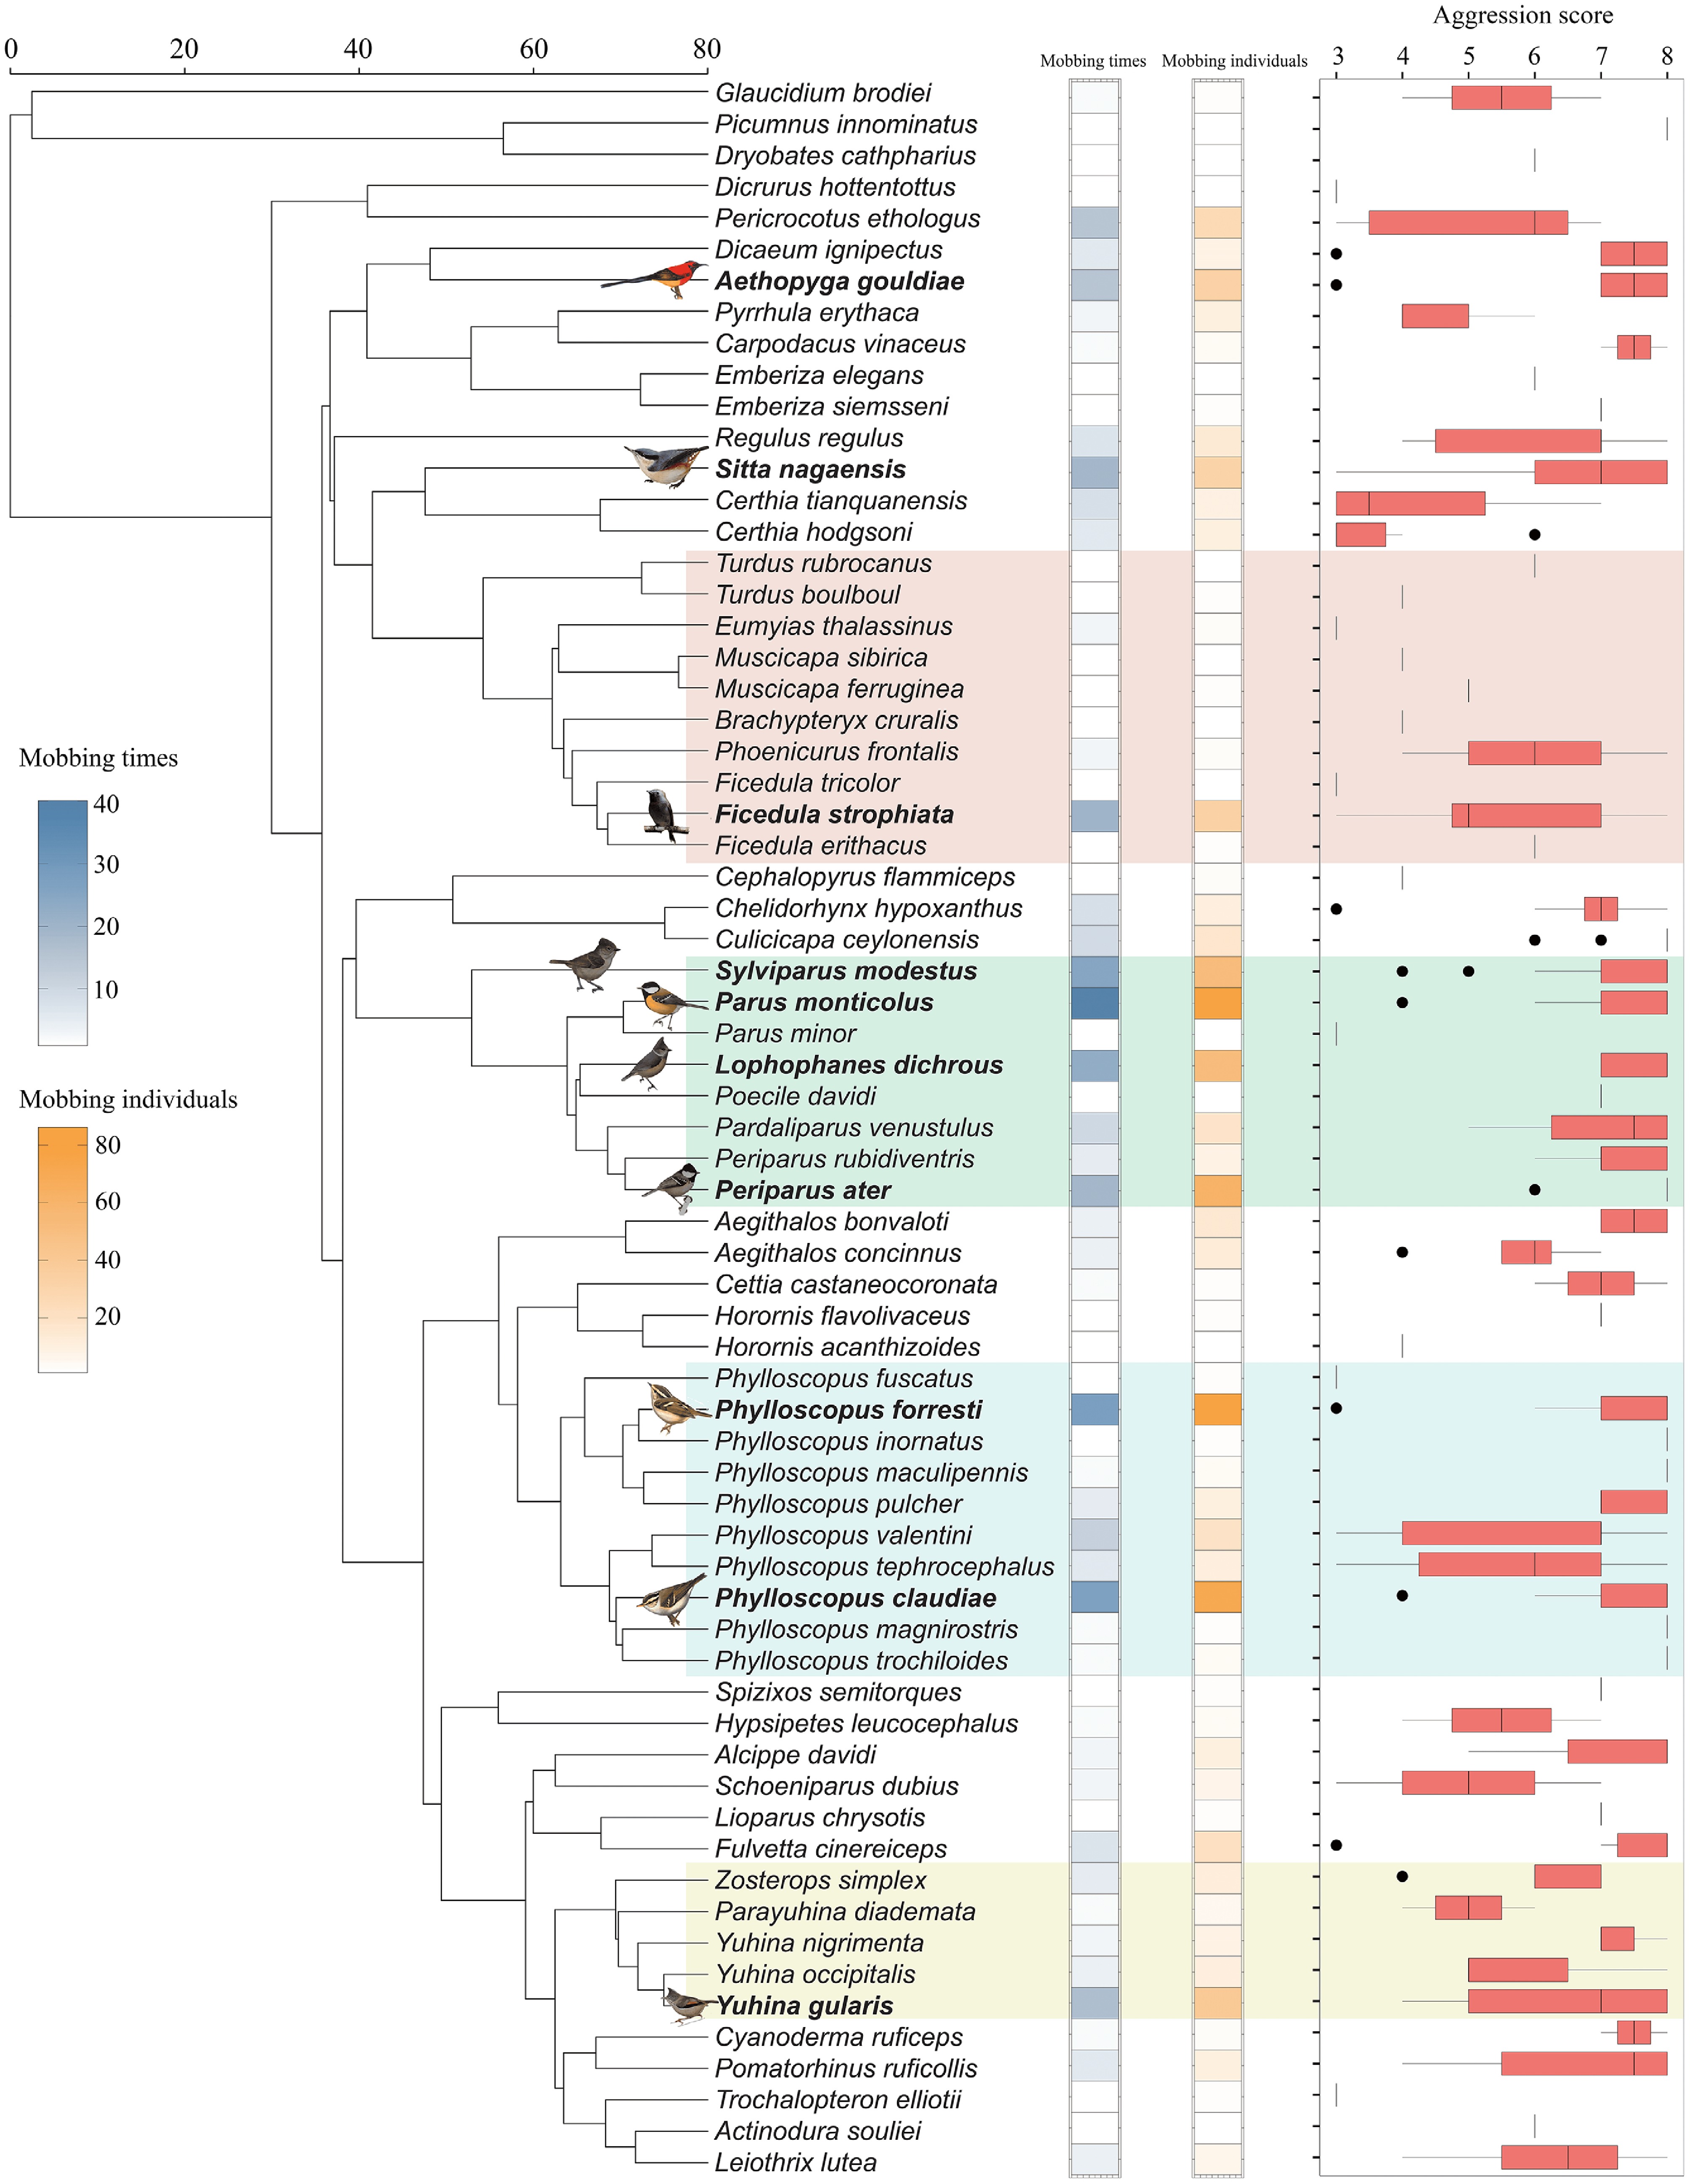
Figure 2.
Phylogenetic relationships and summary of the mobbing status of birds recorded. Boldfaced species are those with mobbing times among the top 10 mobbing birds. The bird images used in this figure were taken from 'The CNG Field Guide to the Birds of China', edited by Yang Liu and Shuihua Chen[36].
Table 1. The mobbing times and individual numbers of the top 10 mobbing bird species.
Species Family Residency
statusMobbing number Mobbing frequency
MFall (%)Mobbing number
of individualsRatio (%) Parus monticolus Paridae R 40 44.44 82 9.15 Phylloscopus forresti Phylloscopidae S 28 31.11 86 9.60 Phylloscopus claudiae Phylloscopidae S 27 30.00 71 7.92 Sylviparus modestus Paridae R 25 27.78 52 5.80 Lophophanes dichrous Paridae R 23 25.56 52 5.80 Ficedula strophiata Muscicapidae S 20 22.22 33 3.68 Sitta nagaensis Sittidae R 19 21.11 31 3.46 Periparus ater Paridae R 19 21.11 62 6.92 Yuhina gularis Zosteropidae R 17 18.89 40 4.46 Aethopyga gouldiae Nectariniidae S 15 16.67 32 3.57 R represents the resident bird, and S represents the summer resident bird. The Jaccard similarity index for mobbing bird communities between different breeding seasons was 34.44%. Of the bird species observed across both breeding seasons, 23 species were consistently present. All of these species belong to the order Passeriformes, with the families Paridae and Phylloscopidae being the most predominant. Six resident species—Green-backed Tit, Grey-crested Tit (Lophophanes dichrous), Coal Tit (Periparus ater), Yellow-browed Tit (Sylviparus modestus), Stripe-throated Yuhina (Yuhina gularis), and Chestnut-vented Nuthatch (Sitta nagaensis)—exhibited high mobbing frequency and number of participating individuals in both seasons. The Green-backed Tit consistently showed the highest mobbing frequency across both breeding and non-breeding seasons, with comparable intensity between seasons (Supplementary Table S3). The Jaccard similarity index for mobbing bird communities between the two elevational bands was 12.99%. Fifteen species, all Passeriformes, were shared between elevational bands. Three species—Green-backed Tit, Claudia's Leaf Warbler (Phylloscopus claudiae), and Stripe-throated Yuhina—demonstrated consistently high mobbing frequency and individual participation across both elevational bands (Supplementary Table S4). The principal behavioral patterns observed included five types: 'mobbing calls + mobbing', 'mobbing calls + hopping', 'mobbing calls + approaching', 'active mobbing', and 'hopping' (Table 2).
Table 2. The probability density of the mobbing indices to the vocalization of the Collared Owlet.
Mobbing indices
(unit, sample size)Peak point
indicator observationsPeak point density (%) The 85% density range of evaluation index Average Lower limit Upper limit Response indices of birds Response time (min, n = 414) 3.26 17.16 4.48 1.31 9.04 Response distance (m, n = 414) 4.88 16.66 4.23 1.20 9.28 Response height (m, n = 414) 3.00 26.23 4.01 1.51 8.53 Aggression score (n = 414) 8.00 41.30 6.92 4.00 8.00 Active layer (n = 414) Understory 48.55 / Ground layer Canopy layer Indices of mobbing assembly The number of participating species (n = 90) 3.00 23.33 4.57 2.00 8.00 The number of participating individuals (n = 90) 5.00 11.11 9.19 3.00 20.00 Assemblage duration (min, n = 89) 6.99 16.65 6.78 2.62 10.06 Mobbing behavior's differences in different elevations and seasons
-
These collective anti-predator events predominantly occurred in the upper-forest layer and lower vertical strata. No significant difference was detected in mobbing formation (presence/absence of assemblages) between breeding seasons (χ2 < 0.001, p = 0.995). However, response duration (t = 4.06, p < 0.001) and assemblage duration (t = 3.11, p = 0.003) were significantly longer during the breeding season, while minimum approach distance was significantly shorter (t = −3.12, p = 0.002). Although the mean number of participating species (t = 1.70, p = 0.094) and individuals (t = 0.91, p = 0.368) per trial was higher in the breeding season, these differences were not statistically significant. No significant seasonal differences were found in mobbing frequency (t = 0.25, p = 0.804) or response height (t = –1.42, p = 0.160), though breeding season responses trended toward higher mobbing frequency and lower vertical positioning. Significant seasonal divergence occurred in behavioral expression (χ2 = 24.53, p < 0.001), with breeding season birds exhibiting higher aggression scores and more offensive behaviors. No significant difference was observed in foraging stratum utilization between seasons (χ2 = 1.80, p = 0.772), with both periods primarily occurring in the understory layer (Fig. 3). Overall, breeding season mobbing assemblages were characterized by larger group sizes and more aggressive behavioral tactics.
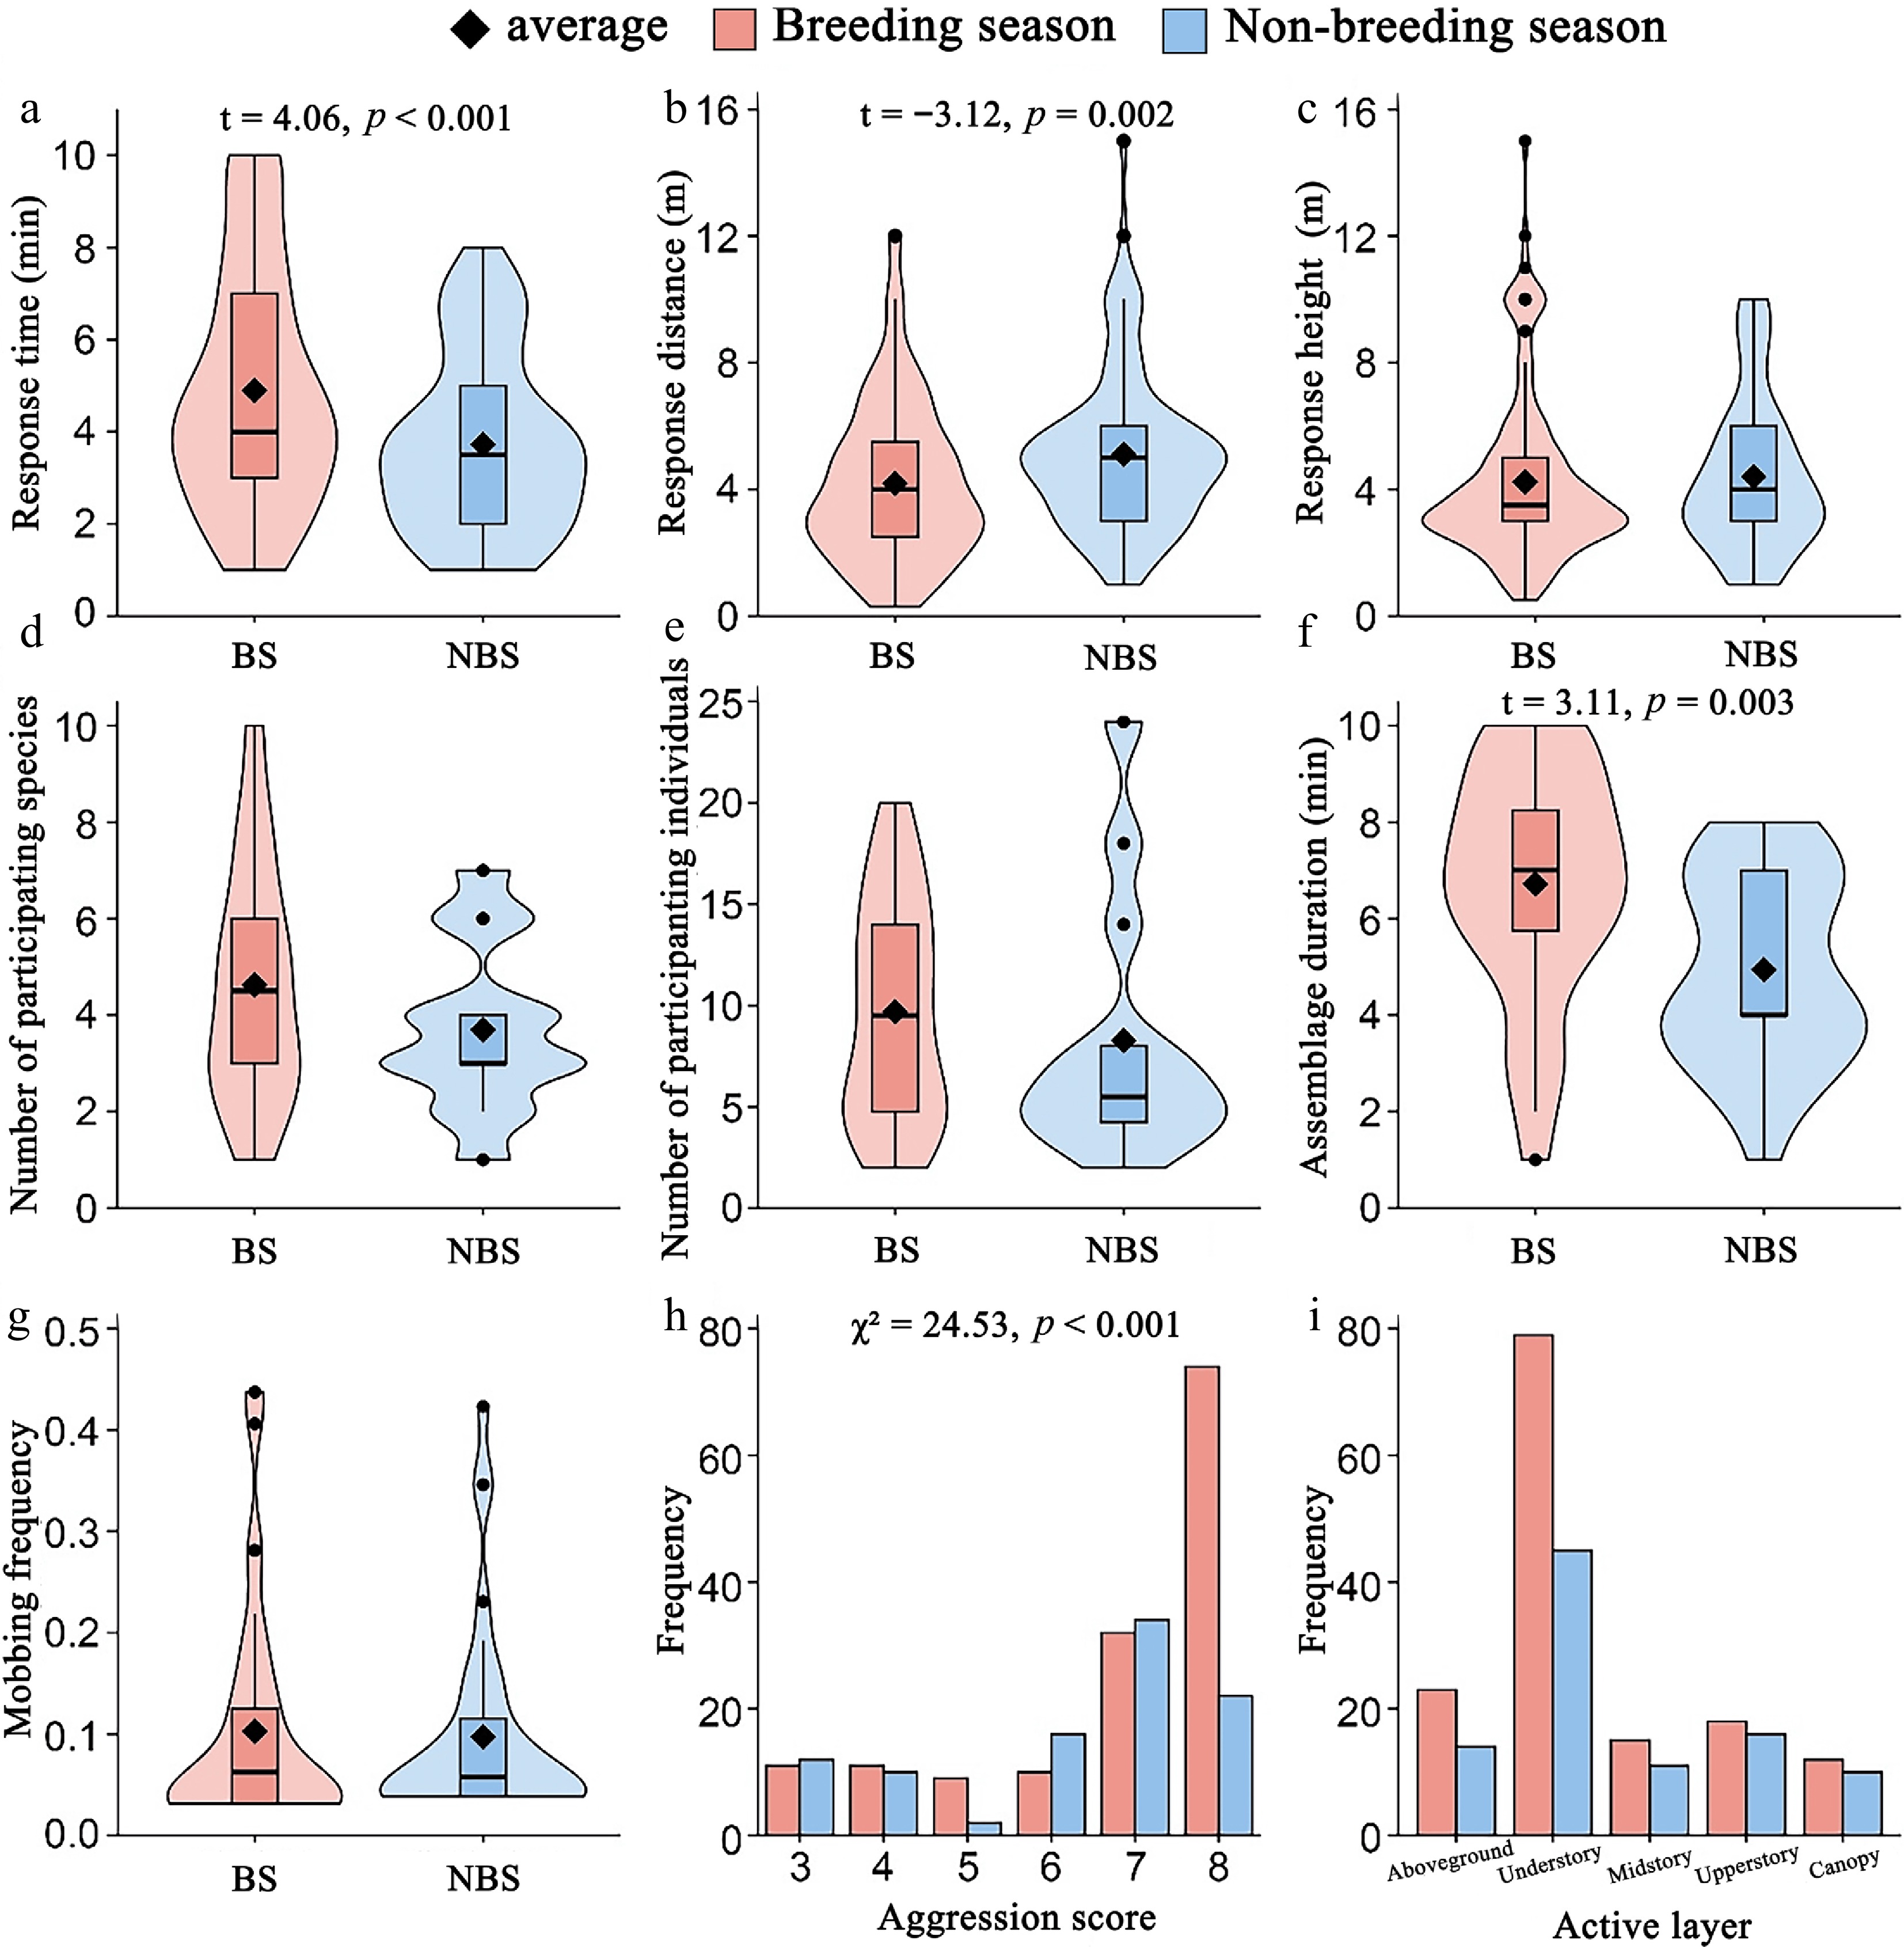
Figure 3.
The mobbing indices to the vocalization of the Collared Owlet in different breeding seasons. BS represents the breeding season, and NBS represents the non-breeding season. (a−g) Comparisons of response time, response distance, response height, number of participating species, number of participating individuals, assemblage duration, and mobbing frequency between breeding season and non-breeding season. (h−i) Distribution of aggression scores and activevegetation layers under different seasons.
The number of valid playback trials was significantly higher in the 2,800–3,200 m elevational band compared to the 1,800–2,200 m band (χ2 = 4.82, p = 0.028), indicating a higher probability of mobbing formation at higher elevations in the primary forest. Birds in the 2,800–3,200 m band exhibited significantly longer response durations (t = −2.49, p = 0.013), higher species richness of participants (t = –3.59, p = 0.001), and a greater total number of responding individuals (t = −3.58, p = 0.001), but significantly lower response heights (t = 2.67, p = 0.008). No significant elevational differences were detected in minimum approach distance (t = 1.74, p = 0.084), mobbing frequency (t = −0.99, p = 0.327), or assemblage duration (t = –1.25, p = 0.214). However, the higher elevational band trended toward higher mean mobbing frequency, longer assemblage duration, and shorter approach distance. Although birds at 2,800–3,200 m displayed higher mean aggression scores, no significant difference in behavioral expression was observed between elevational bands (χ2 = 3.02, p = 0.697). Foraging stratum utilization did not differ significantly between the two bands (χ2 = 9.28, p = 0.054), with both primarily occurring in the understory layer (Fig. 4). On the whole, birds in the 2,800–3,200 m elevational band demonstrated more proactive mobbing participation, formed larger assemblages, and exhibited more aggressive behavioral tactics.
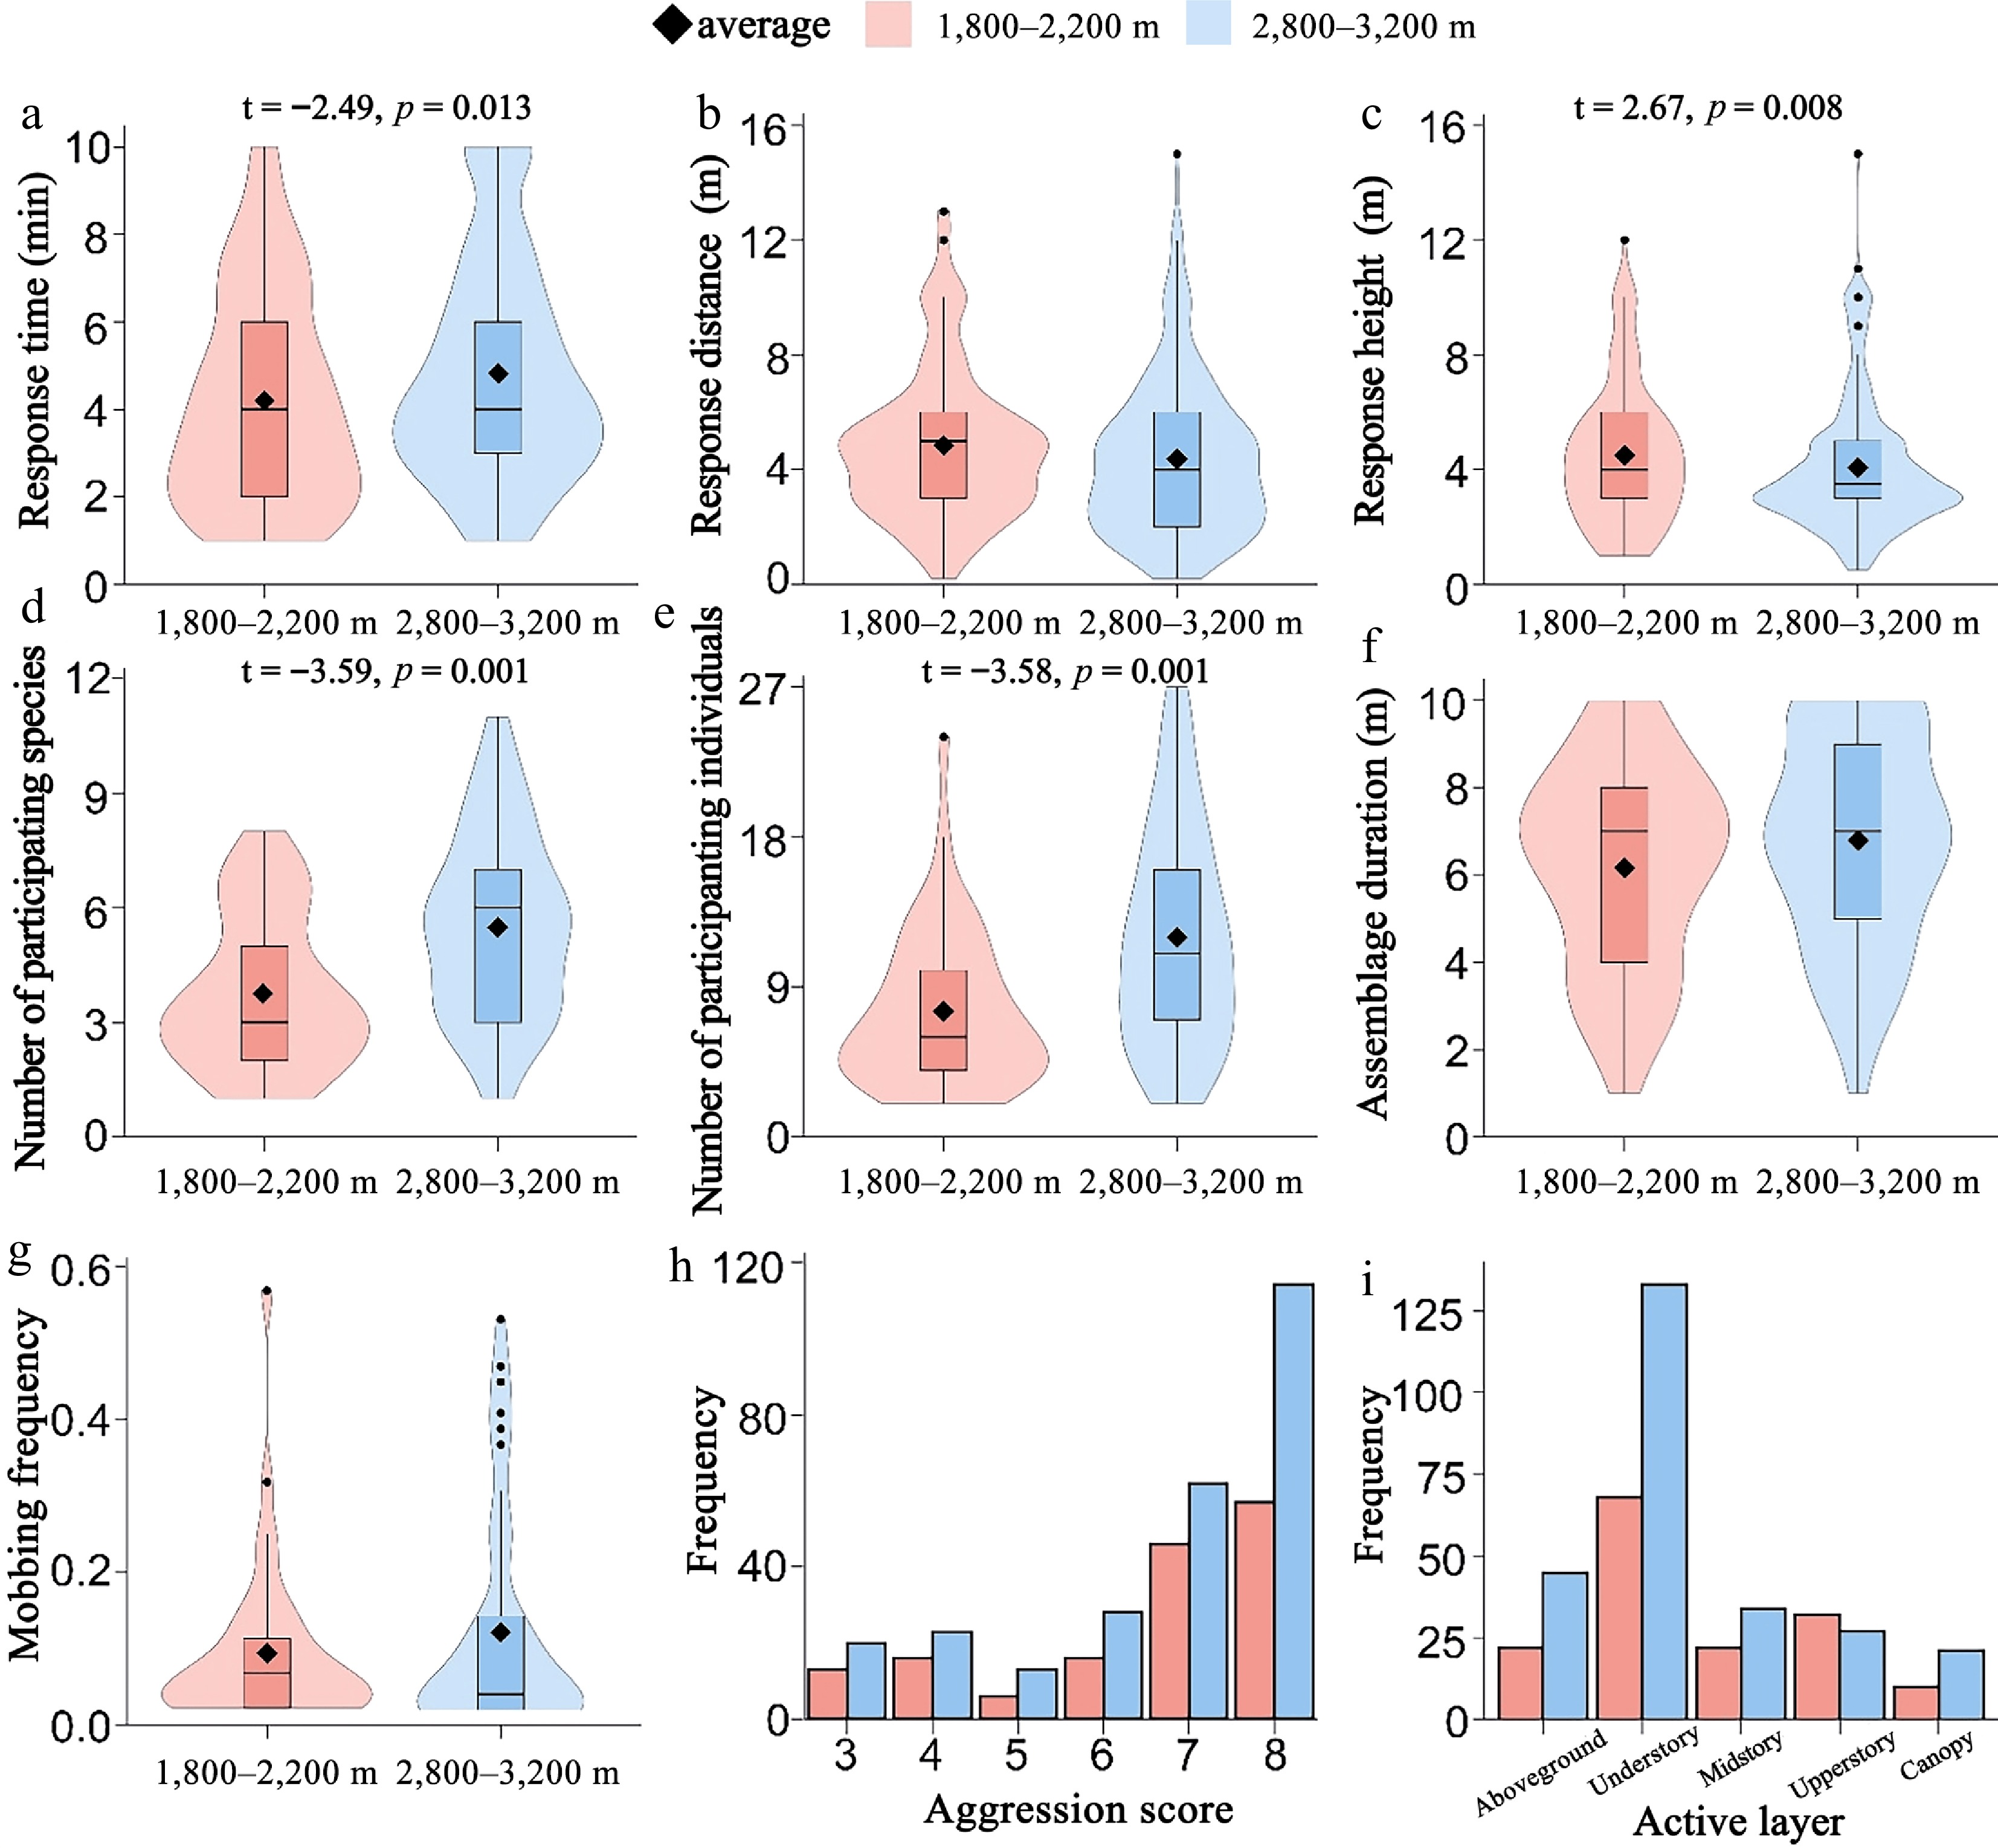
Figure 4.
The mobbing indices to the vocalization of Collared Owlets at different elevations. (a−g) Comparisons of response time, response distance, response height, number of participating species, number of participating individuals, assemblage duration, and mobbing frequency between 1,800-2,200 m and 2,800-3,200 m. (h−i) Distribution of aggression scores and active vegetation layers under different elevations.
Factors influencing avian mobbing behavior
-
Model fitting results revealed that mobbing frequency was significantly negatively correlated with morphological traits (PCA1, representing overall body size) (β = −0.254, p = 0.001), but significantly positively correlated with hand-wing index (β = 0.293, p = 0.030) and species abundance in the study area (β = 0.715, p = 0.001). Additionally, resident birds exhibited significantly higher mobbing times compared to migrants (β = 1.669, p = 0.022) (Supplementary Table S5). After model simplification, the DIC value decreased to 285.946 (ΔDIC = 3.748), and mobbing frequency showed a significant negative correlation with body mass (β = −0.622, p = 0.001) (Fig. 5). The number of participating individuals was significantly negatively correlated with morphological traits (β = −0.284, p = 0.001) and significantly positively correlated with species abundance (β = 0.736, p = 0.001). The hand-wing index had a marginally significant positive effect on participant numbers (β = 0.300, p = 0.056) (Supplementary Table S6). After simplification, the DIC decreased to 330.732 (ΔDIC = 1.565), and participant numbers were significantly negatively correlated with body mass (β = −0.660, 95% CI = [−0.958, −0.367], p = 0.001) (Fig. 5). Mobbing participation was negatively correlated with morphological traits (β = −0.022, 95% CI = [−0.041, −0.004], p = 0.012), indicating that smaller species were more likely to participate, and positively correlated with species abundance (β = 0.159, 95% CI = [0.107, 0.215], p = 0.001). After simplification, the DIC decreased to 14,700.355 (ΔDIC = 16.045), and participation probability was significantly negatively correlated with body mass (β = −0.044, 95% CI = [−0.085, −0.002], p = 0.030) (Fig. 6).
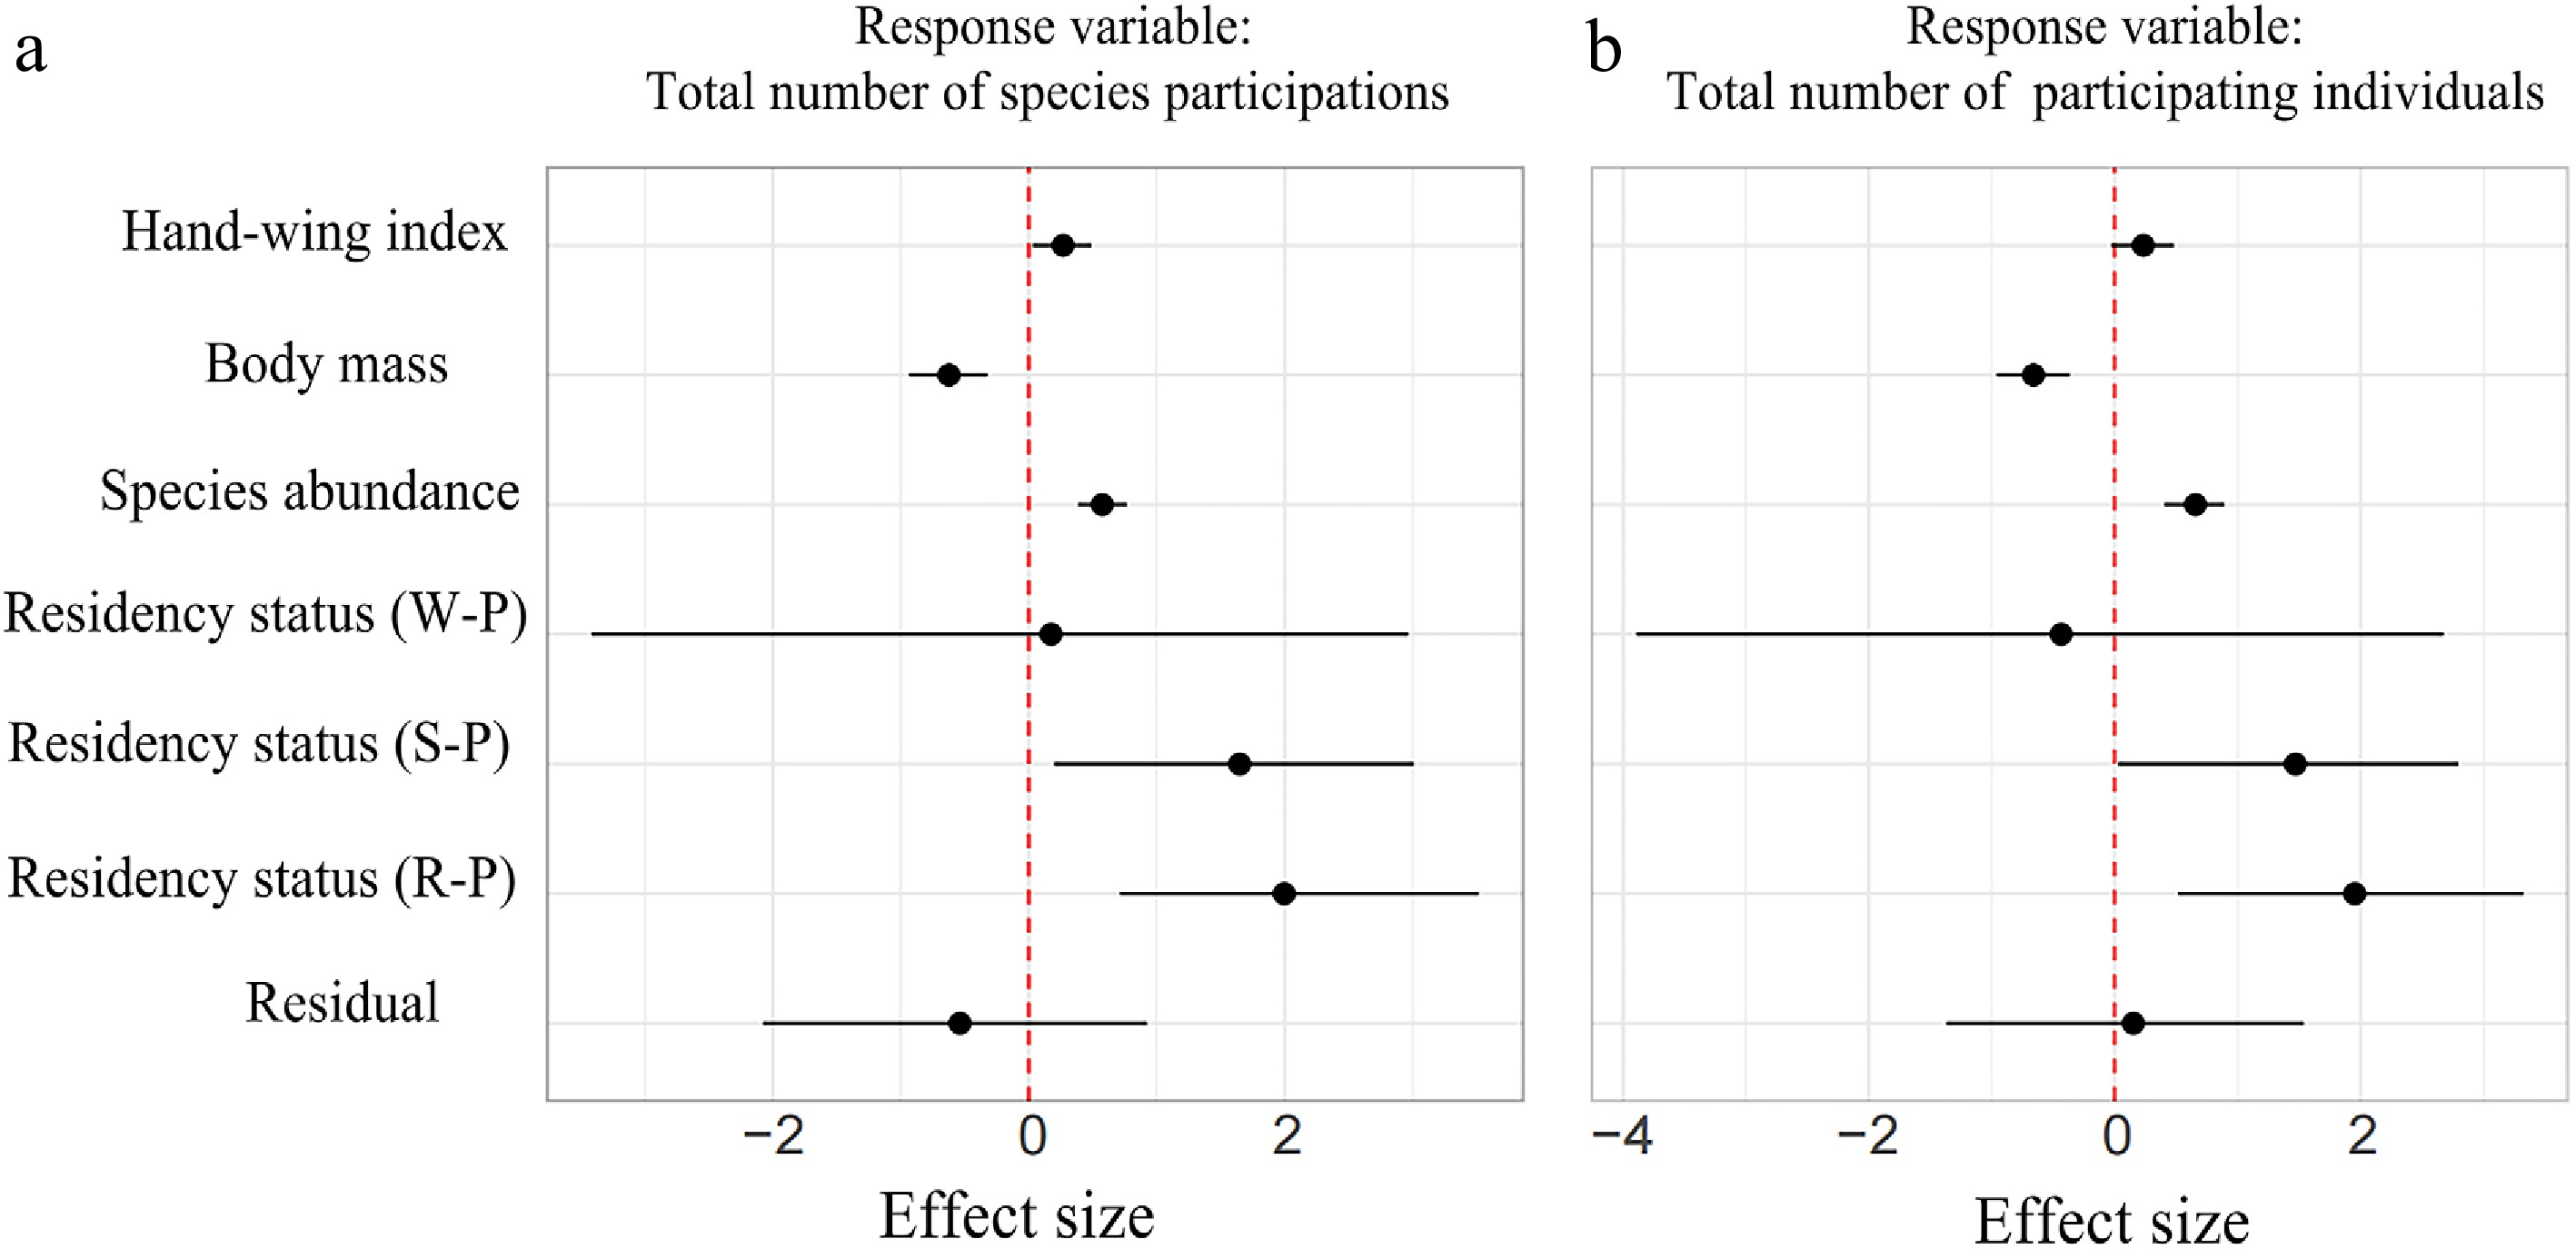
Figure 5.
Fixed effects of the simplified model of mobbing times and individuals of birds with their 95% highest posterior density credible intervals. R represents the resident bird, S represents the summer resident bird, W represents the winter resident bird, and P represents the passing bird; the same below.
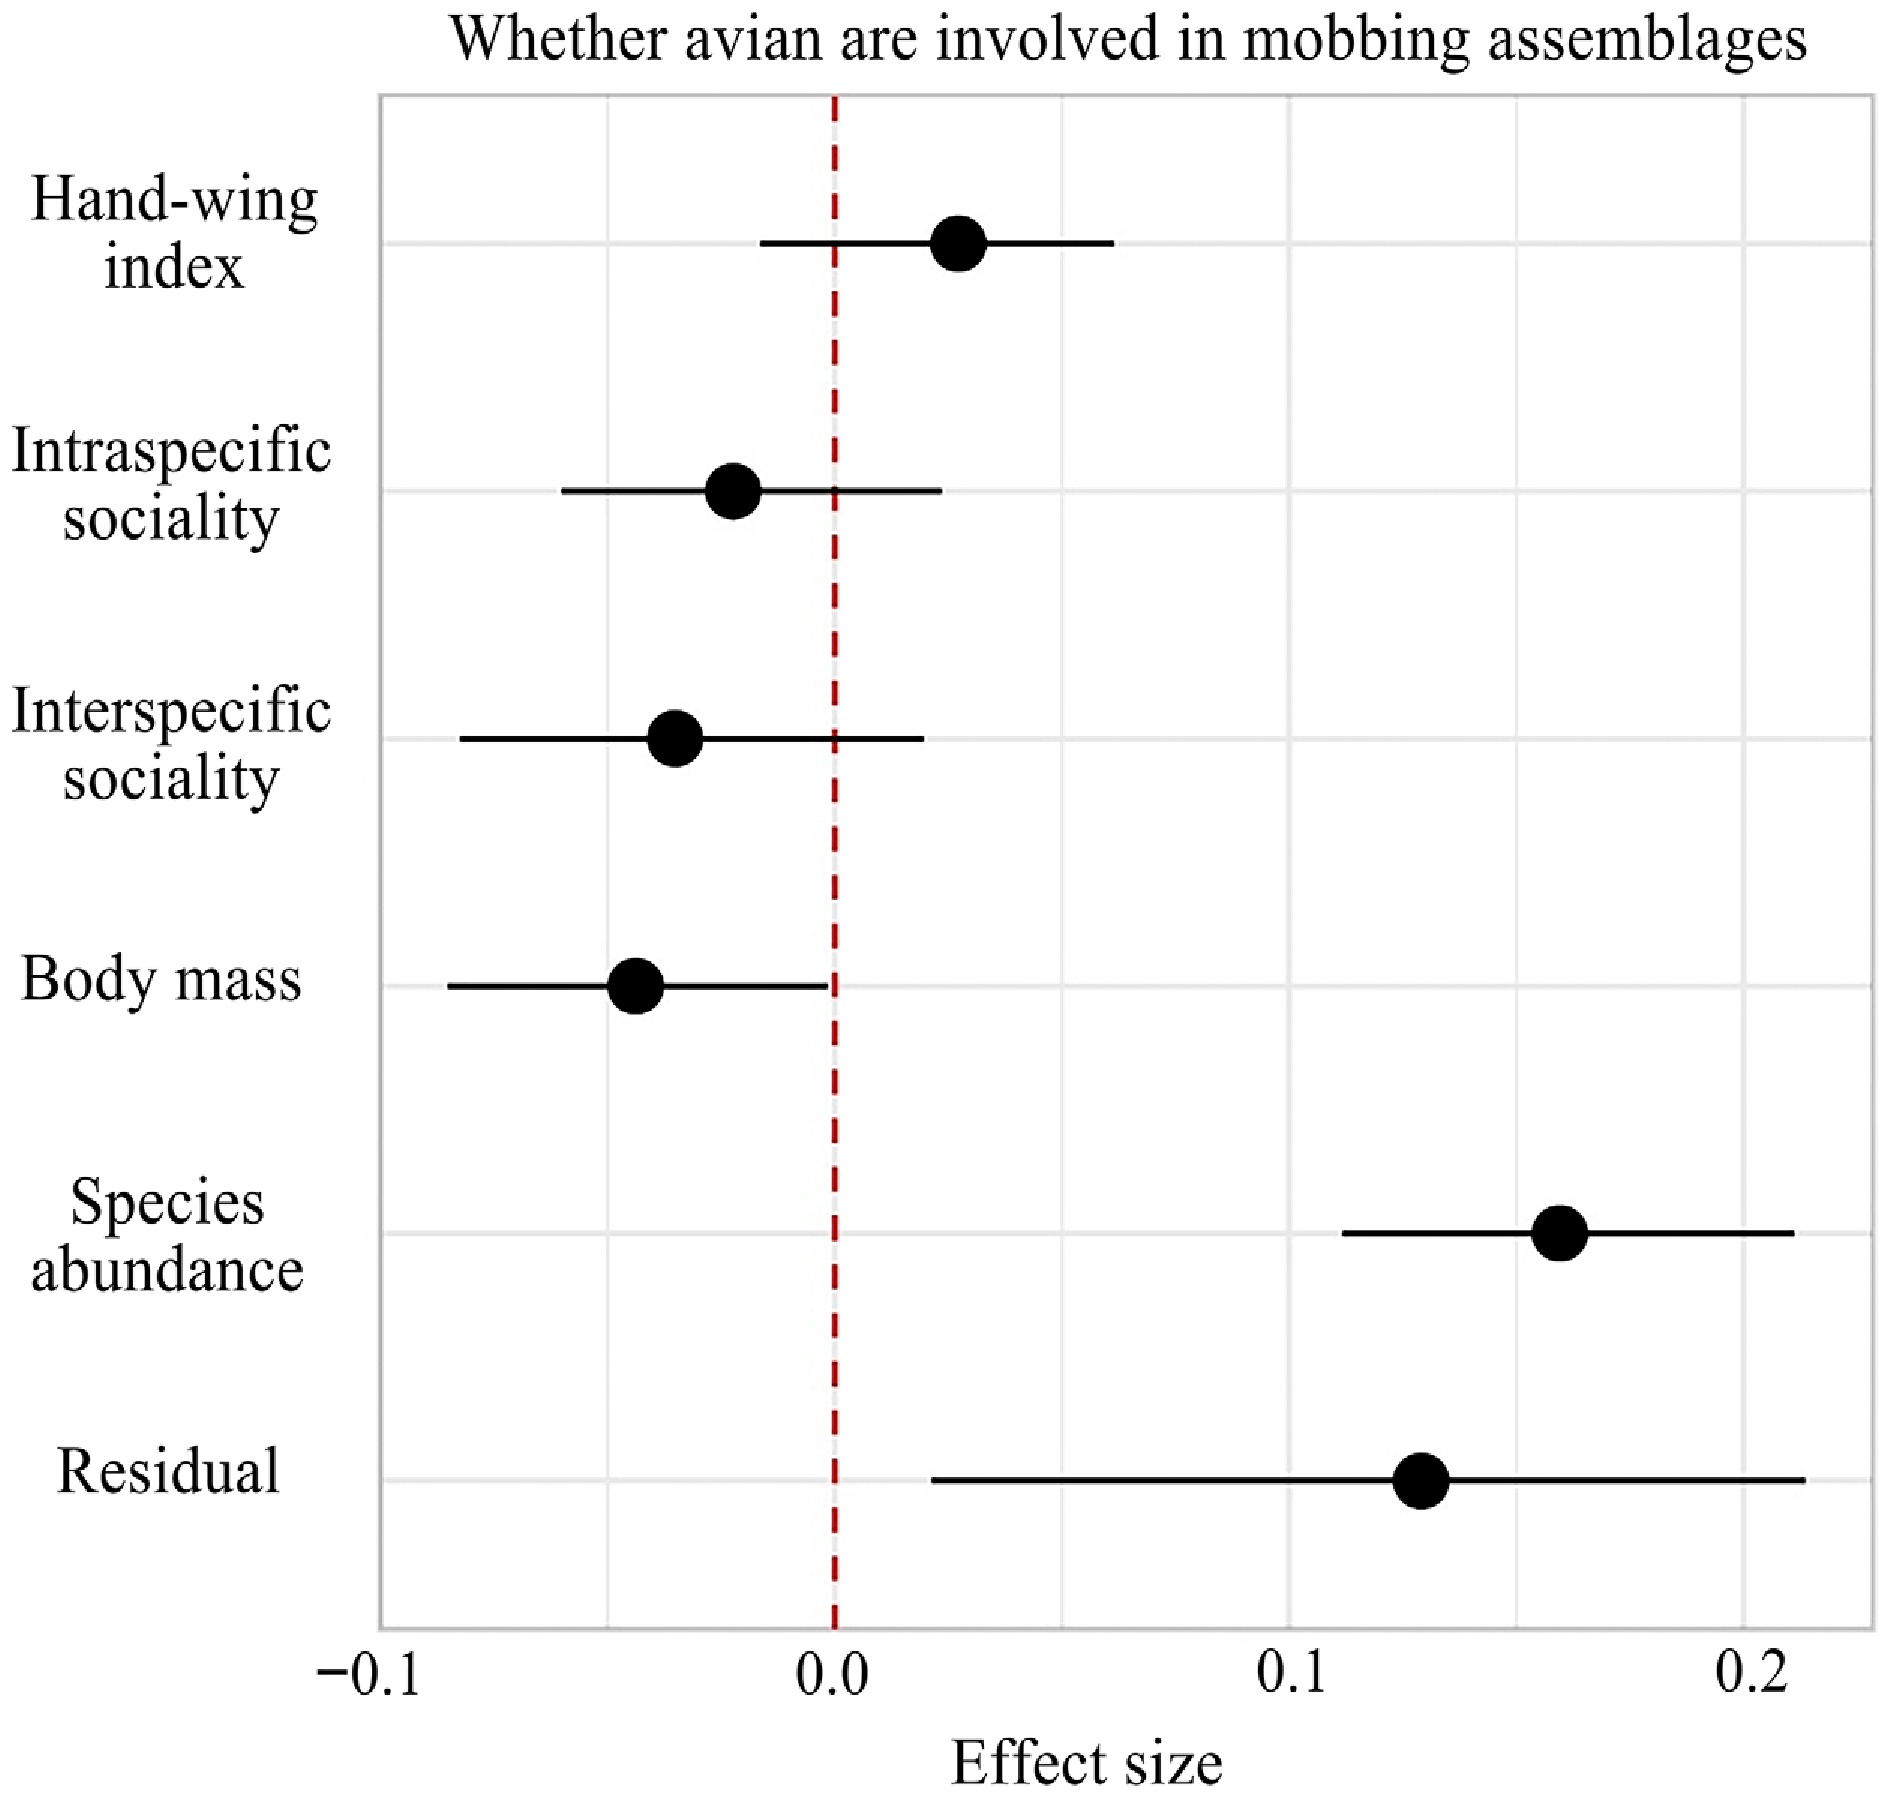
Figure 6.
Fixed effects of the simplified model of mobbing status of birds with their 95% highest posterior density credible interval.
Model results indicated no significant correlation between the number of responding individuals and any predictor variables. However, marginally significant positive correlations were detected with intraspecific sociality (β = 0.128, p = 0.094), and marginally significant negative correlations with foraging height (β = −0.131, p = 0.086) and ambient temperature during playback (β = −0.106, p = 0.055). Response duration was significantly negatively correlated with body mass (β = −0.119, p = 0.035). Compared to the breeding season, birds in the non-breeding season exhibited significantly shorter response durations (β = −0.479, p = 0.002) and significantly larger minimum approach distances (β = 0.389, p = 0.014). Response height was significantly positively correlated with hand-wing index (β = 0.349, p < 0.001) and foraging height (β = 0.157, p = 0.044), but significantly negatively correlated with the first principal component (PC1) of foraging behavior (β = −0.098, p = 0.014) (Table 3). Aggression score was significantly positively correlated with species abundance (β = 0.358, p = 0.011), and showed a marginally significant negative correlation with body mass (β = −0.156, p = 0.052). Compared to the breeding season, non-breeding season birds exhibited significantly lower aggression scores (β = −0.576, p < 0.001) (Table 4).
Table 3. Simplified Bayesian hierarchical model of the relationship between factors and response indices.
Number of responding individuals Response time Response distance Response height β 95% confidence interval p β 95% confidence interval p β 95% confidence interval p β 95% confidence interval p Fixed effects Intercept −0.193 [−0.860, 0.419] 0.534 0.080 [−0.623, 0.789] 0.818 0.134 [−0.690, 0.961] 0.735 0.153 [−0.596, 0.910] 0.665 Body mass −0.081 [−0.196, 0.034] 0.167 −0.119 [−0.229, −0.008] 0.035 0.052 [−0.064, 0.168] 0.375 −0.004 [−0.108, 0.100] 0.940 Foraging behavior
PCA1−0.026 [−0.121, 0.071] 0.591 / / / −0.031 [−0.133, 0.069] 0.548 −0.098 [−0.188, –0.011] 0.029 Hand-wing index 0.066 [−0.086, 0.226] 0.400 / / / 0.102 [−0.067, 0.270] 0.227 0.349 [0.200, 0.500] < 0.001 Foraging height −0.131 [−0.291, 0.018] 0.086 / / / 0.107 [−0.061, 0.273] 0.204 0.157 [0.005, 0.305] 0.044 Intraspecific sociality 0.128 [−0.022, 0.282] 0.094 / / / / / / / / / Temperature −0.106 [−0.213, 0.002] 0.055 −0.085 [−0.211, 0.042] 0.186 / / / −0.091 [−0.231, 0.051] 0.208 Humidity / / / / / / 0.039 [−0.098, 0.173] 0.566 / / / Breeding season
(non-breeding season–breeding season)/ / / −0.479 [−0.771, −0.180] 0.002 0.389 [0.082, 0.702] 0.014 / / / Random effects Phylogenetic relationship 0.475 [0.248, 0.750] / 0.552 [0.345, 0.812] / 0.662 [0.419, 0.968] / 0.600 [0.314, 0.932] / Experiment number 0.191 [0.014, 0.370] / 0.434 [0.296, 0.583] / 0.450 [0.322, 0.589] / 0.578 [0.461, 0.713] / Residual 0.927 [0.855, 1.004] / 0.801 [0.736, 0.873] / 0.773 [0.710, 0.843] / 0.660 [0.604, 0.721] / Table 4. Simplified Bayesian hierarchical model of the relationship between factors and aggressive score.
Response behavior score β 95% confidence interval p Fixed effects Residual 1 −1.953 [−3.236, −0.733] 0.003 Residual 2 −1.330 [−2.592, −0.119] 0.033 Residual 3 −1.088 [−2.352, 0.119] 0.077 Residual 4 −0.633 [−1.874, 0.580] 0.300 Residual 5 0.243 [−0.995, 1.465] 0.679 Body mass −0.156 [−0.321, 0.001] 0.052 Species abundance 0.358 [0.086, 0.654] 0.011 Humidity −0.079 [−0.214, 0.056] 0.253 Breeding season (non-breeding season–breeding season) −0.576 [−0.894, −0.263] < 0.001 Random effects Phylogenetic relationship 1.048 [0.702, 1.500] Experiment number 0.174 [0.008, 0.397] Bold text represents factors that are significantly/marginally significantly correlated to bird response behavior scores. -
Mobbing assemblages were predominantly composed of small-bodied birds. In our study, over 86% of responding birds had a body mass ratio of less than 50% relative to the Collared Owlet. It is a small-sized raptor and demonstrates a pronounced predation preference for small bird species[12]. Furthermore, small bird species typically pose a relatively low physical threat to predators. To effectively drive away a predator, they often need to increase their behavioral investment, such as by emitting mobbing calls with higher frequency and longer duration[37,38]. The relative body size of birds compared to predators influences mobbing efficacy. Specifically, larger-bodied bird species are more effective at altering predator behavior through collective attacks[39]. Overall, small birds derive greater net benefits from collective mobbing. Flight capability, quantified by the hand-wing index, positively influenced mobbing participation[25]. Higher hand-wing indices indicate superior escape ability from potential predator attacks. This suggests that mobbing participation is not arbitrary but reflects a risk assessment based on individual capabilities. Moreover, the active participation of highly capable fliers in mobbing provides greater benefits in reducing predation risk for other birds[15,29].
Higher mobbing frequency and more intense behavioral responses occurred during the breeding season, and in the 2,800–3,200 m elevational band
-
We found that during the breeding season, mobbing birds exhibited a shorter response distance, alongside higher response times and behavioral intensity scores. This heightened response is likely driven by immediate fitness benefits, such as protecting themselves and their offspring. Furthermore, mobbing assemblages in the breeding season have greater species richness, larger group sizes, and longer event durations. Contrary to findings reported by Dagan & Izhaki[16], our study found no increase in mobbing participation during the non-breeding season. This discrepancy may be attributed to the relatively low proportion of winter migrants in our study area, which is not a major overwintering site for birds. The departure of summer migrants likely reduced local avian diversity during the non-breeding season. Our findings revealed no significant difference in mobbing responses between the 2,800–3,200 m elevation range (where Collared Owlets are extremely rare or absent as a resident breeder) and the 1,800–2,200 m range (where they are present). At higher altitudes, the acquisition of mobbing behavior in birds may be facilitated by species capable of altitudinal migration. These individuals potentially lead local bird communities in mobbing events. Specifically, birds with prior experience may train high-elevation communities to recognize and respond to owlet vocalizations. On one hand, in Mt. Gongga, there is a high degree of connectivity and species replacement between adjacent elevational zones[40]. On the other hand, birds can rapidly generalize alarm calls with similar acoustic features. The ability to mob in response to vocalizations of allopatric predators requires acquisition through social learning[41,42].
Previous studies have focused on horizontal spatial variation in avian mobbing behavior, while elevational effects remain poorly explored[7,41]. Habitat and topographic heterogeneity likely drive differences in mobbing patterns across elevational bands. The 1,800–2,200 m band has steep terrain dominated by valley landscapes, where ravines and sand cliff slopes obstruct horizontal acoustic transmissions. This reduces signal detection probability and increases travel time to the sound source. In contrast, the 2,800–3,200 m band has gentler topography, enabling more efficient horizontal sound propagation. Additionally, in the 2,800–3,200 m altitudinal band, the structurally complex understory of the primary coniferous forests at this elevation provides physical conditions conducive to intensified mobbing clusters[16], including diverse vertical perches and concealed horizontal perches closer to the acoustic source. Notably, the Collared Owlet occurs in the 1,800–2,200 m band and vocalizes at dusk or night with calls similar to our playback stimuli. Birds in this band may exhibit habituation to these calls, reducing their acoustic sensitivity to owlet vocalizations.
Parids is a nucleus species in mobbing assemblages
-
This study reaffirmed the role of Parids as proactive mobbing participants and newly identified Green-backed Tit as a hyper-aggressive mobbing species. Despite extensive research on Parids as frequent and vigorous responders in forest mobbing assemblages[43−45], the behavioral profile of the Green-backed Tit remained poorly quantified. Traditionally characterized as a follower species in mixed-species flocks, its role in mobbing had been overlooked[46,47]. We documented 40 mobbing events by Green-backed Tits, which substantially exceeded the second-ranked species, the Sichuan Leaf Warbler (28 events). The Green-backed Tit showed high mobbing frequency and intense response behaviors across both breeding and non-breeding seasons, as well as across elevational gradients. We hypothesize that its ecological dominance and elevated predation risk drive this hyper-vigilance. Green-backed Tit is primarily distributed in Southwestern China, and it is a dominant species in our study area[19]. Bibi et al.[18] documented three cases of Green-backed Tit predation by Collared Owlets within artificial nest boxes in the Zixi Mountains of Yunnan Province, China. These observations provide empirical evidence that Collared Owlets exert direct predation pressure on the Green-backed Tit. Increased predation risk is known to elevate mobbing participation, as higher predator density or attack frequency selects for enhanced anti-predator vigilance[48]. While Pawlak et al.[49] found that the most active and abundant species did not necessarily initiate mobbing, we propose that the Green-backed Tit may play a keystone role in interspecific information transfer during mobbing events.
The number of individuals participating in mobbing and ambient temperature have a negative correlation
-
Playback experiments conducted during both morning and afternoon periods revealed no significant effect of time of day on bird participation in mobbing events. There was also no influence on the intensity of their behavioral responses[14]. We also found a marginally significant negative correlation between the number of responding individuals per event and ambient temperature during experiments. Elevated temperatures impair birds' ability to discriminate conspecific and heterospecific vocalizations and alter their behaviors[50−51]. For example, elevated ambient temperatures reduce the intensity of mobbing behavior in Great Tits (Parus major) and simultaneously impair their foraging efficiency[17,52]. As temperature decreases, birds experience increased metabolic rates and urgent energetic demands. Although individuals under high energy constraints are theoretically expected to be more risk-prone and invest less in individual vigilance, these harsh conditions strongly drive conspecific and heterospecific birds to aggregate into cohesive foraging clusters[53]. Crucially, the resulting increase in flock size triggers the many-eyes effect and the dilution effect, which substantially enhances collective anti-predator vigilance while reducing individual predation risk[54]. This collective safety margin effectively offsets the costs of anti-predator defense, thereby facilitating more frequent and active participation in mobbing assemblages during colder periods.
-
Overall, our results demonstrate that avian mobbing assemblages on Mt. Gongga are structured by the combined effects of species identity, functional traits, and environmental context. Parids, particularly the Green-backed Tit, played a central role in initiating and sustaining collective responses, while participation was predominantly associated with small body size and a higher hand-wing index. Mobbing responses also varied with season, elevation, residency status, and ambient temperature, indicating that both ecological conditions and species-specific characteristics shape collective anti-predator behavior. These findings suggest that mobbing is an emergent community-level process rather than the product of a single behavioral or environmental driver. Predator vocalizations may therefore function as important information cues that promote interspecific communication and coordinated defense, providing a useful framework for understanding avian communication networks across heterogeneous forest environments.
We thank Faming Liu and Quan Lan at the Gongga Alpine Ecosystem Observation and Research Station for their kind assistance with the fieldwork. Thanks to the Gongga Mountain National Nature Reserve for their help and support. We also thank the editor and the anonymous reviewers for their careful evaluation and constructive feedback, which greatly improved the quality, clarity, and theoretical integration of this study.
-
All procedures in this experiment were conducted following the National Wildlife Conservation Law (https://en.npc.gov.cn.cdurl.cn/2022-12/30/c_1085104.htm), and with permission from the Forestry Department of Ganzi Tibetan Autonomous Prefecture.
-
The authors confirm their contributions to the paper as follows: validation, investigation: Zhang J, Guo J, Wang Y; methodology, investigation, data curation, visualization: Yang Z; writing − original draft, visualization, methodology, conceptualization: Fu S; design, writing − review and editing, supervision, funding acquisition, conceptualization: Wu Y. All authors reviewed the results and approved the final version of the manuscript.
-
Data are available as Supplementary information. We downloaded 5,000 pseudo-posterior distribution trees encompassing all responding bird species from http://birdtree.org. Morphological traits were obtained from the Life-history and Ecological Traits Database of Chinese Birds.
-
The authors declare the following financial interests/personal relationships that may be considered as potential competing interests: Yongjie Wu reports that financial support was provided by the National Natural Science Foundation of China. The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
-
accompanies this paper online at: https://doi.org/10.48130/jzser-0026-0010.
-
# Authors contributed equally: Shijia Fu, Zhixiong Yang
- Supplementary Table S1 The aggression score of mobbing birds.
- Supplementary Table S2 List of birds responding to playback experiments in the study area.
- Supplementary Table S3 The mobbing times and individual number of the top ten mobbing bird species in different breeding seasons.
- Supplementary Table S4 The mobbing times and individual number of the top ten mobbing bird species at different elevations.
- Supplementary Table S5 MCMC GLMM analysis of the relationship between factors and mobbing times of species.
- Supplementary Table S6 MCMC GLMM analysis of the relationship between factors and mobbing individuals of species.
- Supplementary Fig. S1 Heat map of correlation of continuous variable.
- Copyright © 2026 by the author(s). Journal of Zoological Systematics and Evolutionary Research published by Maximum Academic Press on behalf of John Wiley & Sons Ltd. This is an open access article under the terms of the Creative Commons Attribution License, which permits use, distribution and reproduction in any medium, provided the original work is properly cited.
-
About this article
Cite this article
Fu S, Yang Z, Zhang J, Guo J, Wang Y, et al. 2026. Avian mobbing in different seasons and elevations: a playback experiment at Mt. Gongga. Journal of Zoological Systematics and Evolutionary Research 2026: e009 doi: 10.48130/jzser-0026-0010 

Avian mobbing in different seasons and elevations: a playback experiment at Mt. Gongga
- Received: 02 April 2026
- Revised: 03 July 2026
- Accepted: 07 August 2026
- Published online: 04 September 2026
Journal of Zoological Systematics and Evolutionary Research
2026,
Article number: e009 (2026)
|
Cite this article
Abstract: Vocalization is an effective way that birds use to communicate. Rapid recognition of acoustic signals and behavioral responses is crucial for the survival and reproductive success of birds. Understanding how prey species respond to predator calls is important to understanding the avian community communication network. We played the sound of the Collared Owlet (Taenioptynx brodiei) in the forest habitats of eastern Mt. Gongga and compared differences in the response of avian communities in different seasons and elevations. We explored determinants of mobbing behavior at both species and community levels by integrating phylogenetic relationships, functional traits, and environmental factors. We found that mobbing assemblages were dominated by Passerines, with Paridae contributing the highest species richness and abundance. Interestingly, Green-backed Tit (Parus monticolus) was the most frequent and numerous participant, which was the primary initiator of collective anti-predator responses. Mobbing events were primarily driven by small-bodied bird species, and participation showed a positive correlation with the hand-wing index. Higher mobbing frequency and more intense behavioral responses occurred during the breeding season and in the 2,800–3,200 m elevational band. Additionally, resident birds exhibited significantly higher mobbing times compared to migrants. We also found a marginally significant negative correlation between the number of mobbing individuals and the ambient temperature. This study improved our understanding of anti-predator strategies of birds and set up an example for exploring the avian community communication network in other regions of the world.
-
Key words:
- Mobbing behavior /
- Anti-predation strategies /
- Mt. Gongga /
- Playback experiment /
- Community interaction