







-
Oil palm (Elaeis guineensis Jacq.) is a perennial tropical woody oil crop belonging to the Arecaceae family. It is the most efficient oil-producing crop worldwide, with palm oil accounting for approximately one-third of global vegetable oil production[1]. The fruit mesocarp and kernel yield palm oil and palm kernel oil, which are widely used in food processing, industrial manufacturing, and biofuel production[2]. Despite its economic importance, oil palm breeding remains challenging due to its long life cycle (10–15 years from seed to maturity), large plant size, and complex genetic background. Conventional hybridization has made limited progress in developing high-yielding and stress-tolerant varieties, particularly for cultivation in marginal environments such as the northern tropical regions of China[3]. Therefore, the development of efficient genetic transformation systems is urgently needed to accelerate molecular breeding and gene function studies in oil palm.
Tissue culture has been established as a powerful tool for clonal propagation of oil palm, enabling large-scale production of uniform planting materials[4]. Embryogenic callus derived from various explants, including immature zygotic embryos, leaves, and inflorescences, has been successfully used for plant regeneration[5,6]. However, the regeneration process is time-consuming, often taking 12–18 months from callus induction to plantlet acclimatization, and the efficiency remains highly genotype-dependent[7]. To overcome these limitations, genetic transformation approaches have been explored to introduce beneficial genes that promote cell proliferation, somatic embryogenesis, and shoot regeneration. Among various transformation methods, Agrobacterium-mediated transformation offers several advantages, including low transgene copy number, stable integration, and cost-effectiveness[8]. Although oil palm is a monocot and not a natural host for Agrobacterium, successful transformations have been reported using embryogenic callus as explants, with transformation efficiencies typically below 1%[9,10]. Optimization of key parameters such as bacterial concentration, infection duration, acetosyringone (AS) concentration, and co-cultivation time is therefore critical for improving transformation efficiency in recalcitrant species like oil palm[11].
Growth-regulating factors (GRFs) are plant-specific transcription factors that play essential roles in regulating cell proliferation, organ growth, and development. The GRF protein family is characterized by two highly conserved domains at the N-terminus: the QLQ domain (Gln-Leu-Gln), which mediates interaction with GRF-interacting factors (GIFs), and the WRC domain (Trp-Arg-Cys), which is responsible for DNA binding and nuclear localization[12,13]. Since the first identification of OsGRF1 in rice, GRF family members have been characterized in numerous plant species, including Arabidopsis[12], soybean[14], sorghum[15], and birch[16]. GIFs are transcriptional co-activators that lack DNA-binding activity but contain an SNH (SSXT) domain that enables interaction with GRFs and recruitment of chromatin remodeling complexes[17,18]. The GRF-GIF complex has been shown to promote cell proliferation and organ expansion by activating downstream target genes involved in cell cycle regulation[19]. Overexpression of GRFs has been reported to increase leaf size in Arabidopsis[12], Chinese cabbage[20], and lettuce[21], while GRF-GIF co-expression has been demonstrated to enhance regeneration efficiency in multiple crops. Notably, Debernardi et al.[22] showed that a chimeric GRF-GIF fusion protein significantly improved transformation efficiency and regeneration capacity in wheat, rice, and citrus, providing a promising strategy for recalcitrant plant species.
Despite the established roles of GRF and GIF genes in plant growth and regeneration, their functions in oil palm have not been systematically characterized. In this study, we performed genome-wide identification and characterization of the EgGRF and EgGIF gene families in oil palm. Based on transcriptome and qPCR analyses, we identified candidate genes that are highly expressed in regenerable callus. We then optimized key parameters of Agrobacterium-mediated transformation using oil palm embryogenic callus as explants. Finally, we evaluated the effects of single and co-expression of EgGRF1, EgGRF7, and EgGIF3 on transformation screening efficiency and callus differentiation rate. The results demonstrate that EgGRF1-EgGIF3 co-expression significantly enhances transformation screening efficiency and differentiation capacity at the callus/embryogenic stage, providing an optimized protocol and valuable gene resources for functional studies in oil palm.
-
Embryogenic calli of oil palm (Elaeis guineensis Jacq.) were provided by the Coconut Research Institute, Chinese Academy of Tropical Agricultural Sciences (CATAS). Calli were subcultured monthly on maintenance medium (MS basal medium with appropriate hormones, pH 5.8) at 25 ± 2 °C in the dark. Nicotiana benthamiana plants used for dual-luciferase assays were grown at 25 °C under a 16-h light/8-h dark photoperiod.
Identification and bioinformatic analysis of EgGRF and EgGIF genes
-
The GRF and GIF gene families in oil palm were identified through BLASTP searches (E-value ≤ 1 × 10−40) using query sequences from Arabidopsis thaliana, Oryza sativa, and Zea mays. Conserved domains (QLQ and WRC for GRFs; SSXT for GIFs) were validated using Pfam and SMART. Phylogenetic trees were constructed using MEGA 7.0 with the neighbor-joining method (1,000 bootstrap replicates). Conserved motifs were analyzed using MEME, gene structures using GSDS 2.0, and promoter cis-elements (2,000 bp upstream) using PlantCARE. Chromosomal locations and synteny were analyzed with MCScanX and visualized using TBtools.
Transcriptome sequencing and RT-qPCR
-
Total RNA was extracted from robust regenerable callus (RC) and poorly growing browned callus (PC) using the RNAprep Pure Plant Kit (Tiangen, Beijing). RNA-seq libraries were prepared and sequenced on an Illumina platform. Clean reads were aligned to the oil palm reference genome using HISAT2, and expression levels were quantified as FPKM. For RT-qPCR, first-strand cDNA was synthesized using the TransScript Kit (TransGen, Beijing). qPCR was performed using 2× SYBR Green Master Mix (Takara) on an ABI 7500 FAST system with three biological replicates. The oil palm Actin gene served as the internal control, and relative expression was calculated using the 2−ΔΔCᴛ method.
Dual-Luciferase complementation imaging (LCI) assay
-
The coding sequences of EgGRF1 and EgGRF7 were cloned into the pCAMBIA1300-nLUC vector, and EgGIF3 was cloned into pCAMBIA1300-cLUC. Constructs were transformed into Agrobacterium strain GV3101 (pSoup). Co-infiltrations into N. benthamiana leaves were performed as follows: (++) nLUC-GRF + cLUC-GIF; (+) nLUC-empty + cLUC-GIF; (−) nLUC-empty + cLUC-empty; (−+) nLUC-GRF + cLUC-empty. After 48 h, luciferase activity was detected using a plant living imaging system (Tanon, China).
Vector construction and Agrobacterium transformation
-
The coding sequences of EgGRF1, EgGRF7, and EgGIF3 were amplified from oil palm callus cDNA. For single-gene overexpression, amplicons were cloned into the pNC-Cam1304-MCS35S vector using the NimbleCloning (NC) kit (Nimble, China). For co-expression constructs, EgGRF1 (without a stop codon) and EgGIF3 were fused by overlap extension PCR; the same strategy was used for EgGRF7-EgGIF3. All constructs were confirmed by Sanger sequencing and transformed into Agrobacterium strain EHA105.
For transformation optimization, embryogenic calli were pre-cultured on Murashige and Skoog (MS0) medium for 3–4 d. Agrobacterium suspensions were prepared at OD600 values of 0.4–0.8, and calli were infected for 20–50 min. Acetosyringone (AS) concentrations of 50–250 μmol/L were tested. After infection, calli were co-cultivated at 20 °C for 36–84 h, then washed with timentin (500 mg/L) and placed on selection medium containing 60 mg/L hygromycin B. Subculturing was performed every 3 weeks.
Screening efficiency and differentiation rate
-
Green fluorescent protein (GFP) fluorescence was observed under a LUYOR-3415 excitation light source. Screening efficiency was calculated as (Number of GFP-positive embryoids after 3–4 rounds of selection/Total number of infected calli) × 100. GFP-positive embryoids were identified based on stable fluorescence under a LUYOR-3415 excitation light source. Differentiation rate was calculated as (Number of GFP-positive regenerated shoots derived from embryoids/Total number of GFP-positive embryoids) × 100.
PCR confirmation
-
Genomic DNA was extracted from hygromycin-resistant embryoids using the Plant Genomic DNA Kit (Tiangen, Beijing, China). Embryoids were the primary tissue type used for PCR analysis due to their abundance after selection. Where available, DNA was also extracted from embryogenic calli and regenerated shoots for additional verification, though these materials were limited in quantity. The presence of the hygromycin resistance gene (Hyg) was detected by PCR using specific primers (Hyg-F and Hyg-R). For co-expression constructs, gene-specific primers spanning the fusion junction were used to confirm the presence of the intact fusion gene in transgenic materials at different developmental stages.
Statistical analysis
-
All experiments were performed with three independent biological replicates. Data were expressed as mean ± standard deviation (SD). Statistical analyses were performed using GraphPad Prism 10 software. Comparisons among multiple groups were conducted using one-way ANOVA followed by Tukey‘s multiple comparison test. Differences with p < 0.05 were considered statistically significant, and p < 0.01 (**) or p < 0.0001 (****) were considered highly significant.
-
A total of 14 EgGRF and 4 EgGIF genes were identified in the oil palm genome through genome-wide analysis. The EgGRF proteins ranged from 260 to 605 amino acids in length, with molecular weights from 27.62 to 65.30 kDa and theoretical pI values from 5.88 to 9.28 (Supplementary Table S1). All EgGRF proteins exhibited instability indices above 40 and negative GRAVY values, suggesting that most EgGRF proteins may be unstable under in vitro conditions. The four EgGIF proteins ranged from 191 to 222 amino acids, with molecular weights from 20.15 to 23.85 kDa and pI values below 7.
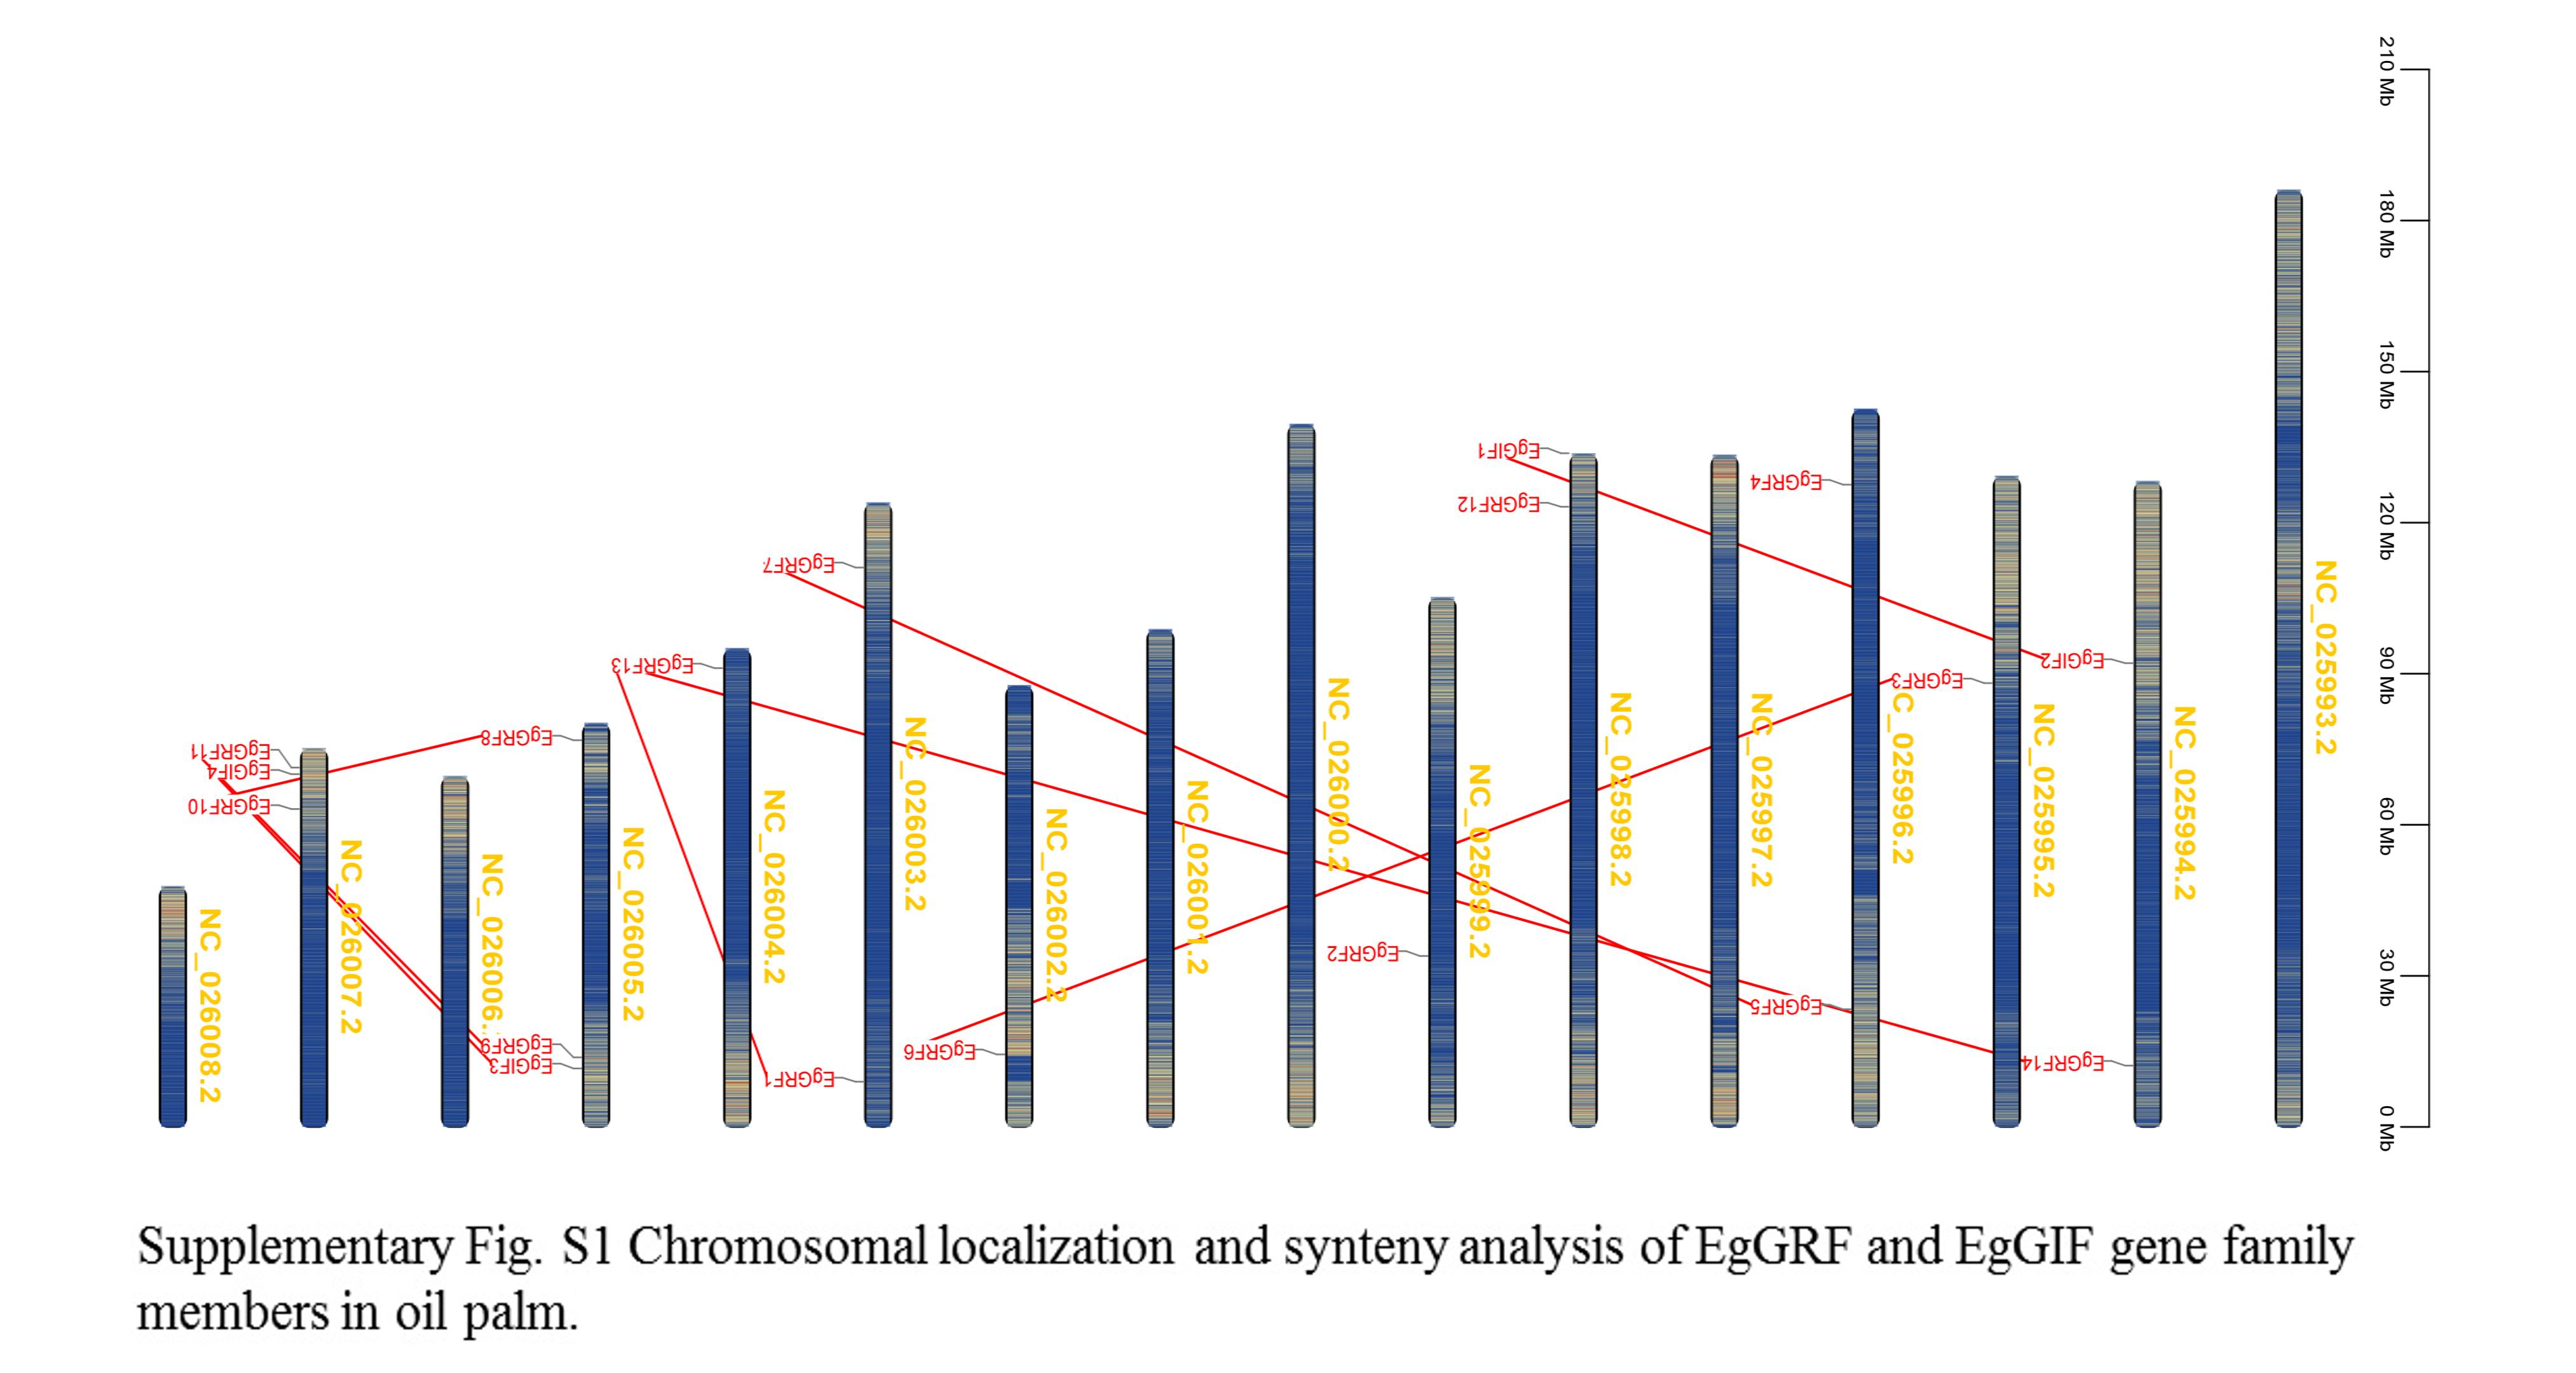
Phylogenetic analysis of GRF proteins from oil palm, Arabidopsis, rice, and maize revealed that all GRF members could be classified into three subfamilies (I, II, and III) (Fig. 1a). Subfamily II contained the largest number of members (23), while subfamily I contained the fewest (8). The 14 EgGRF members were distributed across all three subfamilies. Conserved motif analysis showed that all EgGRF proteins contained the characteristic QLQ and WRC domains (motif1 and motif2), while some members also possessed an additional motif3 (Fig. 1b). All four EgGIF proteins contained the conserved SSXT domain (Fig. 1c). Promoter cis-element analysis revealed that both EgGRF and EgGIF genes harbor multiple elements related to hormone responses (ABRE, TGA-element, P-box), light responses (G-box, I-box, ACE), and stress responses (LTR, TC-rich repeats) (Fig. 1d). Chromosomal localization and synteny analysis indicated that EgGRF and EgGIF genes are distributed across 16 chromosomes, with several segmental duplication events observed (Supplementary Fig. S1).
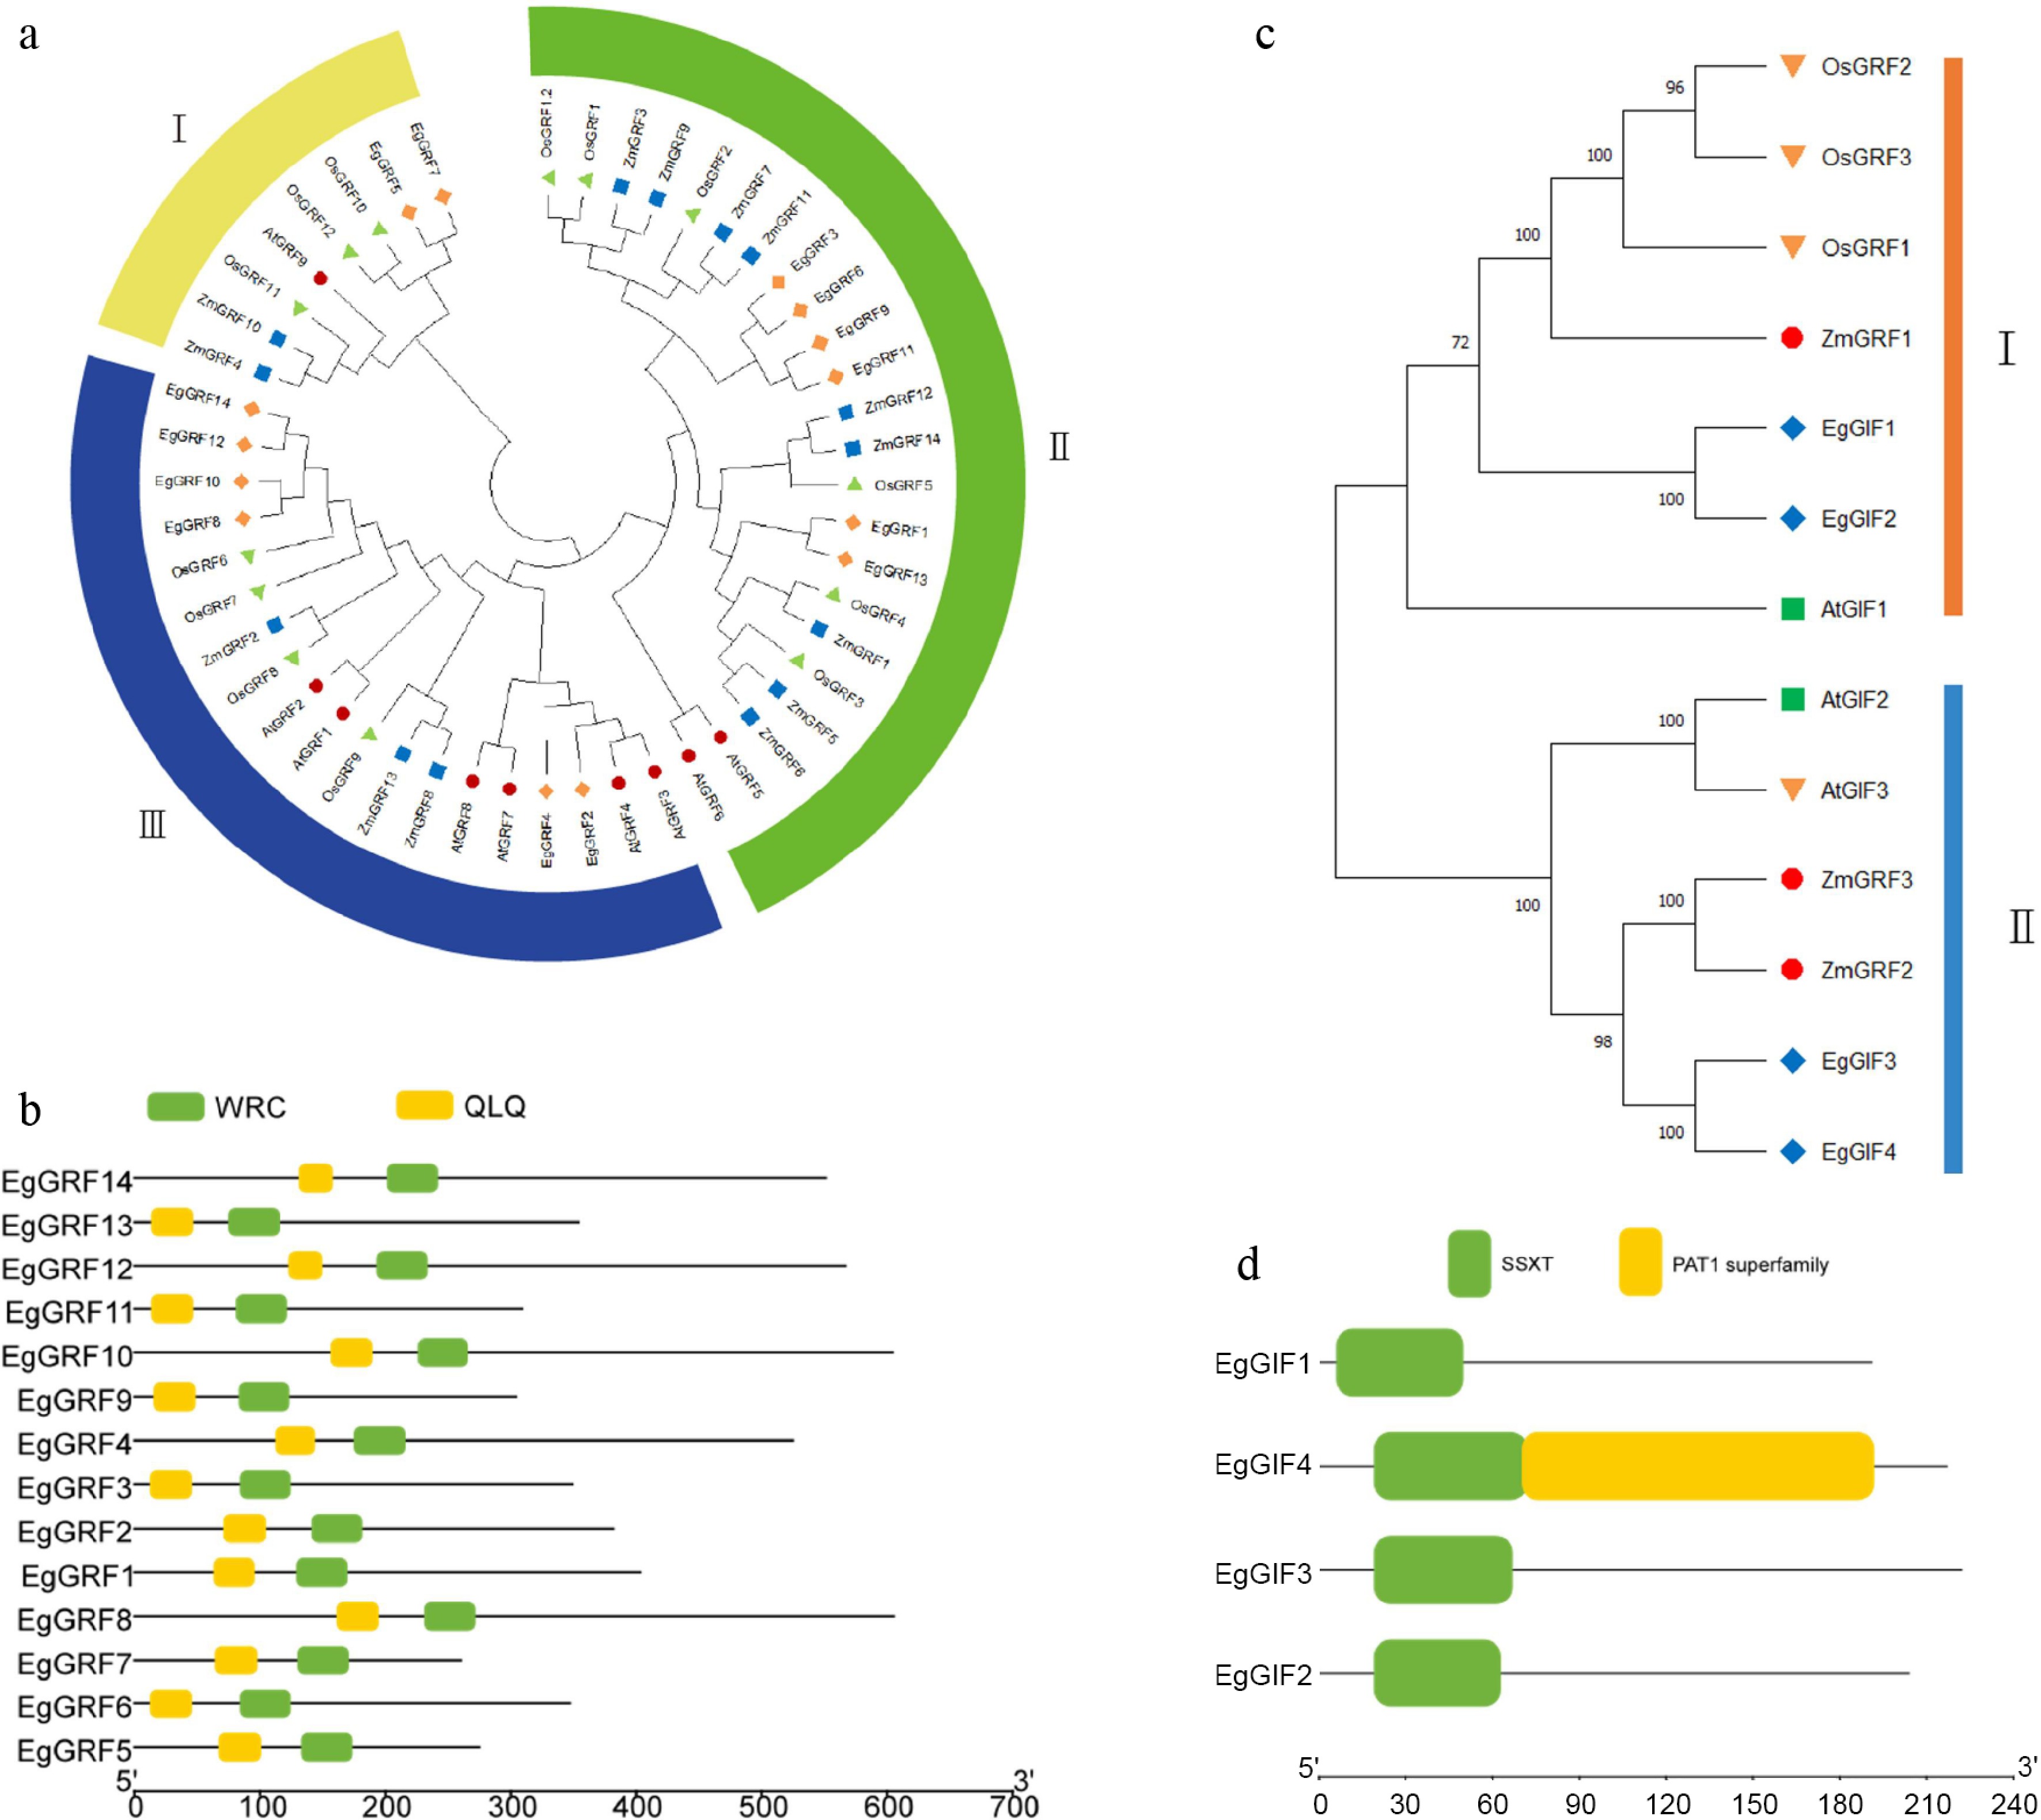
Figure 1.
Phylogenetic relationships and conserved domains of EgGRF and EgGIF genes in oil palm. (a) Phylogenetic tree of the GRF family. (b) Conserved domains of EgGRF family members in oil palm. (c) Phylogenetic tree of the GIF family. (d) Conserved domains of EgGIF family members in oil palm.
Expression patterns of EgGRFs and EgGIFs in different callus types
-
To identify candidate GRF and GIF genes potentially involved in callus proliferation and regeneration, transcriptome sequencing was performed on RC and poorly growing, browned callus (PC) (Fig. 2a). Differential expression analysis revealed that several EgGRF genes, including EgGRF1, EgGRF2, EgGRF3, and EgGRF7, were significantly upregulated in RC compared to PC (Fig. 2b). Among the EgGIF genes, EgGIF2 and EgGIF3 showed significantly higher expression in RC.
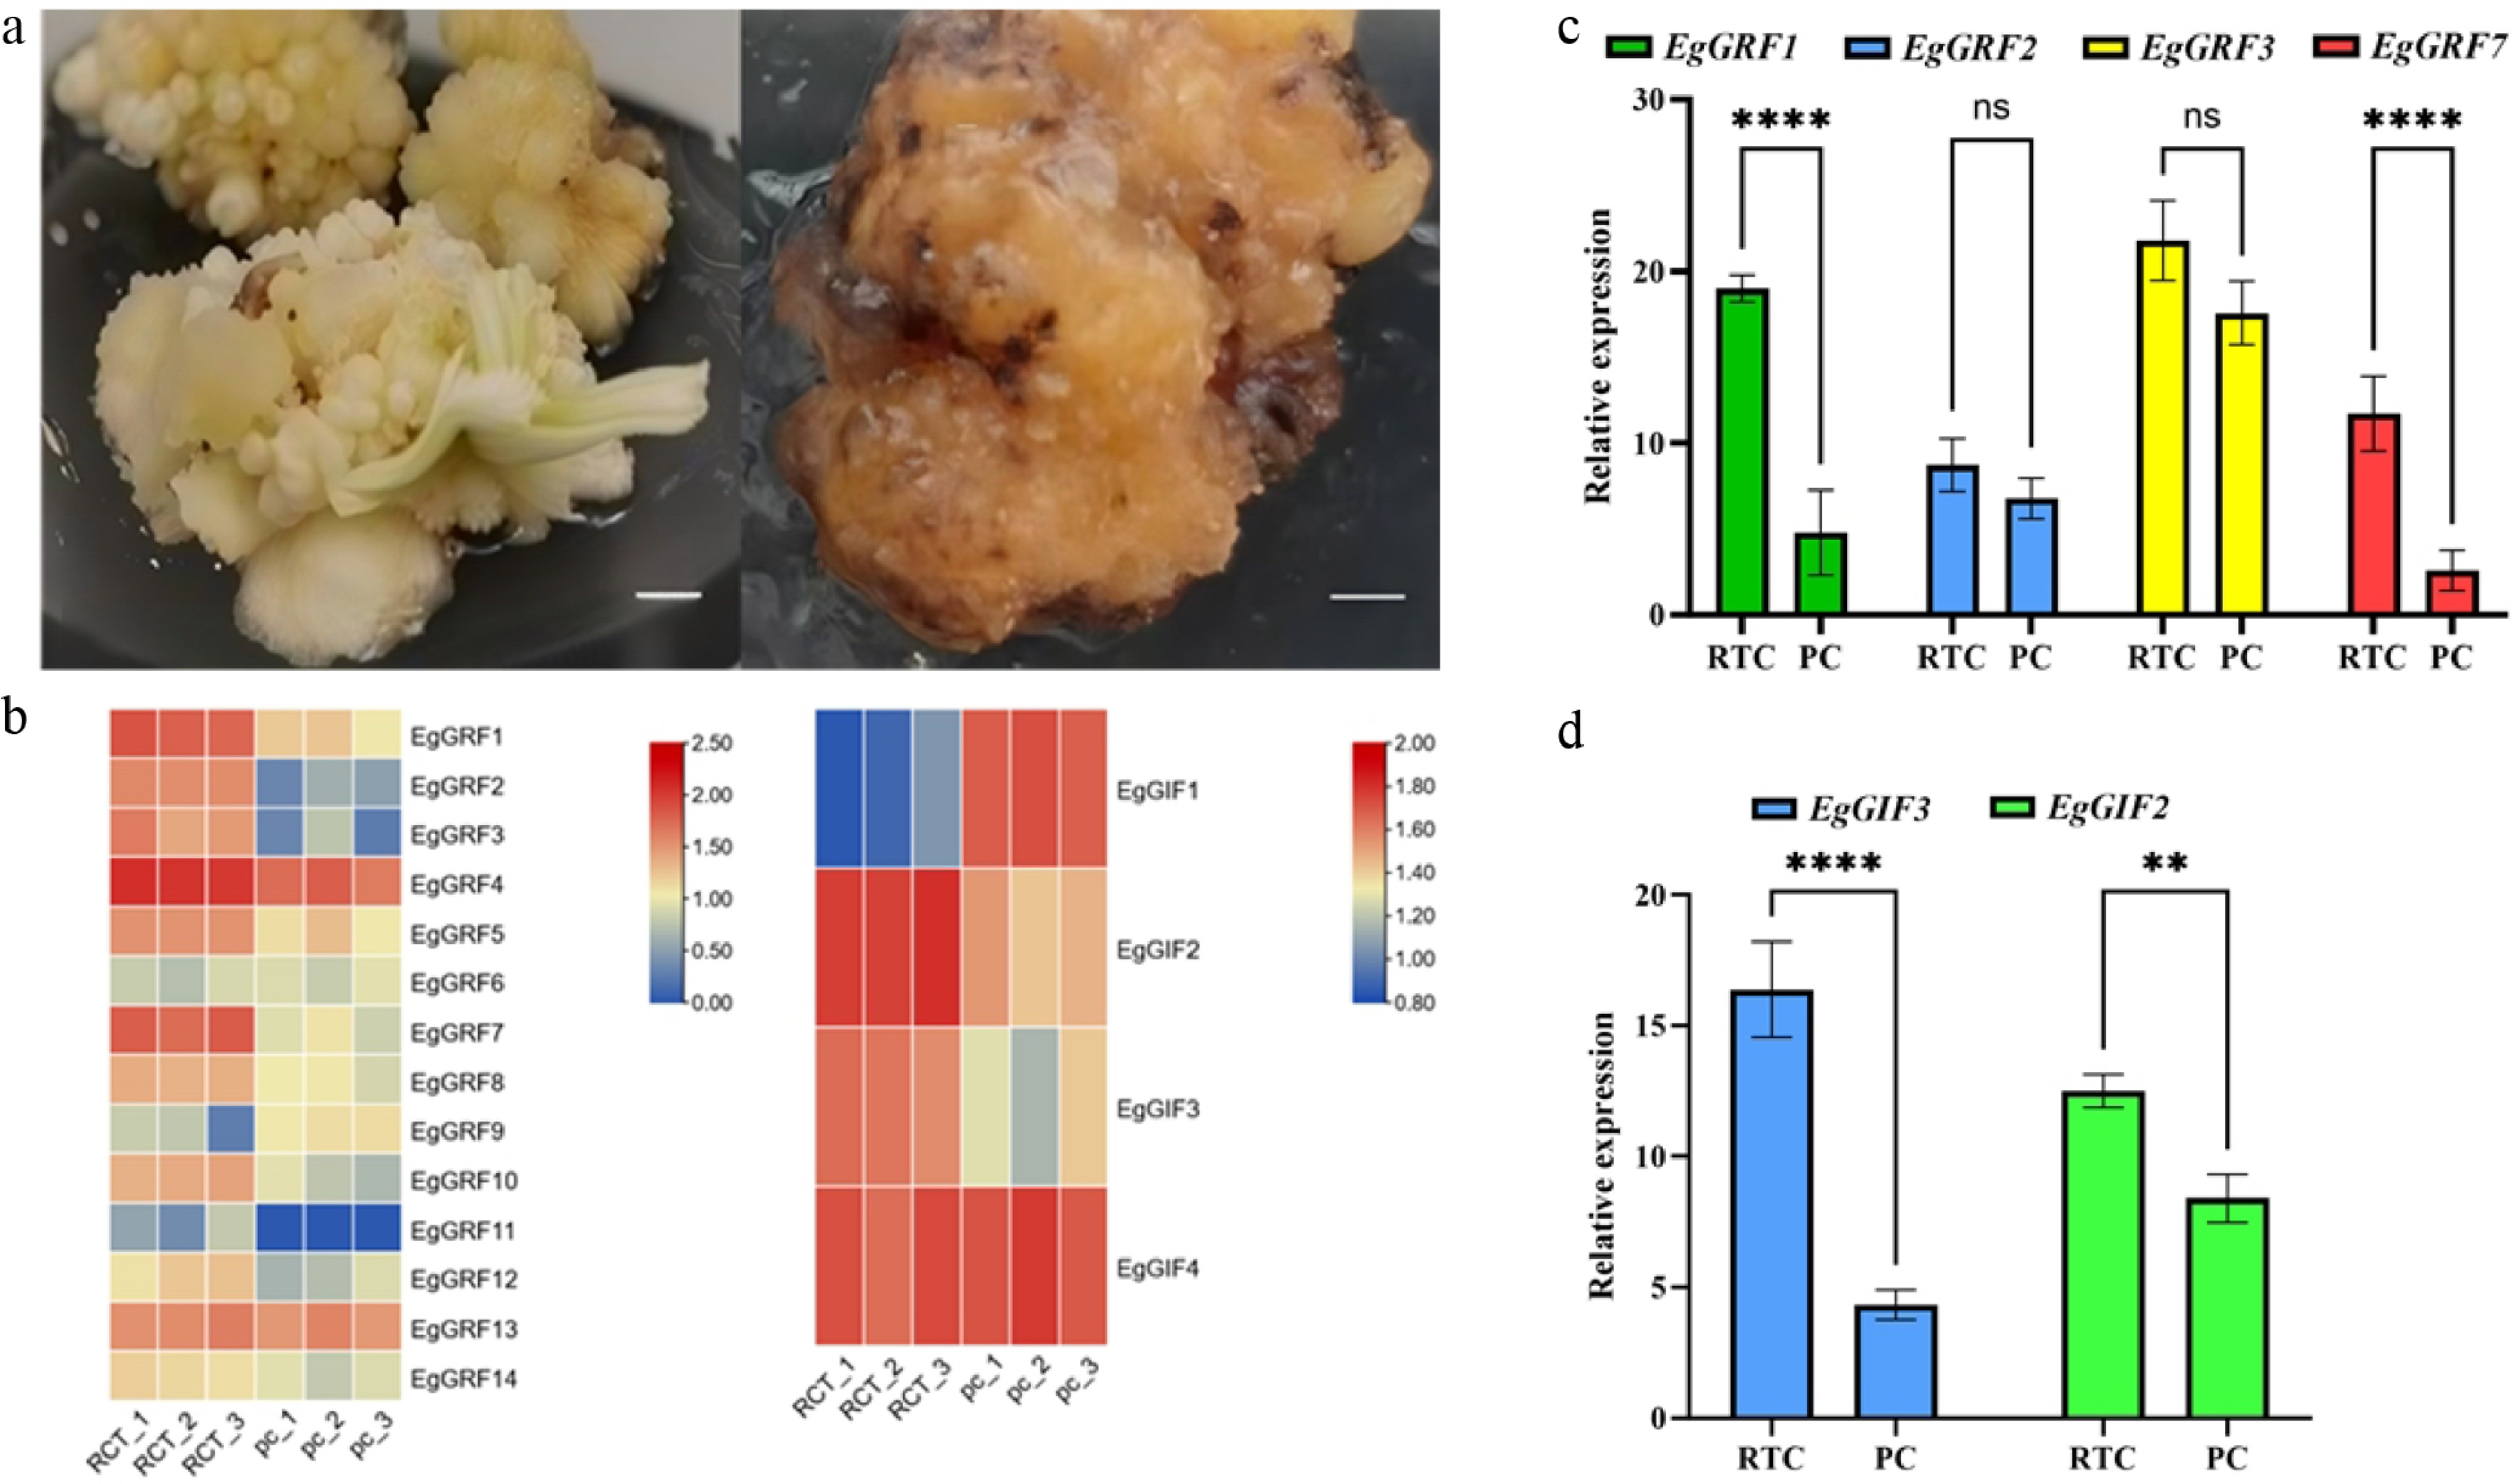
Figure 2.
Differential expression of EgGRF and EgGIF genes between robust regenerable callus (RC) and poorly growing callus (PC). (a) Oil palm callus at different physiological states. Scale bar = 5 mm. (b) Differential expression of oil palm EgGIF and EgGRF genes in callus tissue. (c) Differential expression of GRF genes in oil palm callus. (d) Differential expression of GIF genes in oil palm callus.
RT-qPCR was further performed to validate the transcriptome results. Consistent with the RNA-seq data, EgGRF1 and EgGRF7 exhibited significantly higher expression levels in RC than in PC, with EgGRF1 showing the most pronounced difference (p < 0.0001) (Fig. 2c). In contrast, no significant differences were observed for EgGRF2 and EgGRF3 between the two callus types. Among the GIF genes, EgGIF3 showed highly significant upregulation in RC (p < 0.0001), whereas EgGIF2 showed a significant difference (Fig. 2d). These results suggest that EgGRF1, EgGRF7, and EgGIF3 may play important roles in oil palm callus proliferation and regeneration.
Protein–protein interaction between EgGRF1/EgGRF7 and EgGIF3
-
To investigate whether EgGRF1 and EgGRF7 physically interact with EgGIF3, a dual-luciferase complementation assay (LCI) was performed in N. benthamiana leaves (Fig. 3a, b). Strong luciferase activity was detected when nLUC-EgGRF1 was co-infiltrated with cLUC-EgGIF3 (Fig. 3c). Similarly, co-infiltration of nLUC-EgGRF7 with cLUC-EgGIF3 also produced detectable luminescence (Fig. 3d). In contrast, no luciferase activity was observed in the negative control combinations (empty vectors or single constructs). These results demonstrate that both EgGRF1 and EgGRF7 can physically interact with EgGIF3 in plant cells, providing a molecular basis for their potential synergistic function.
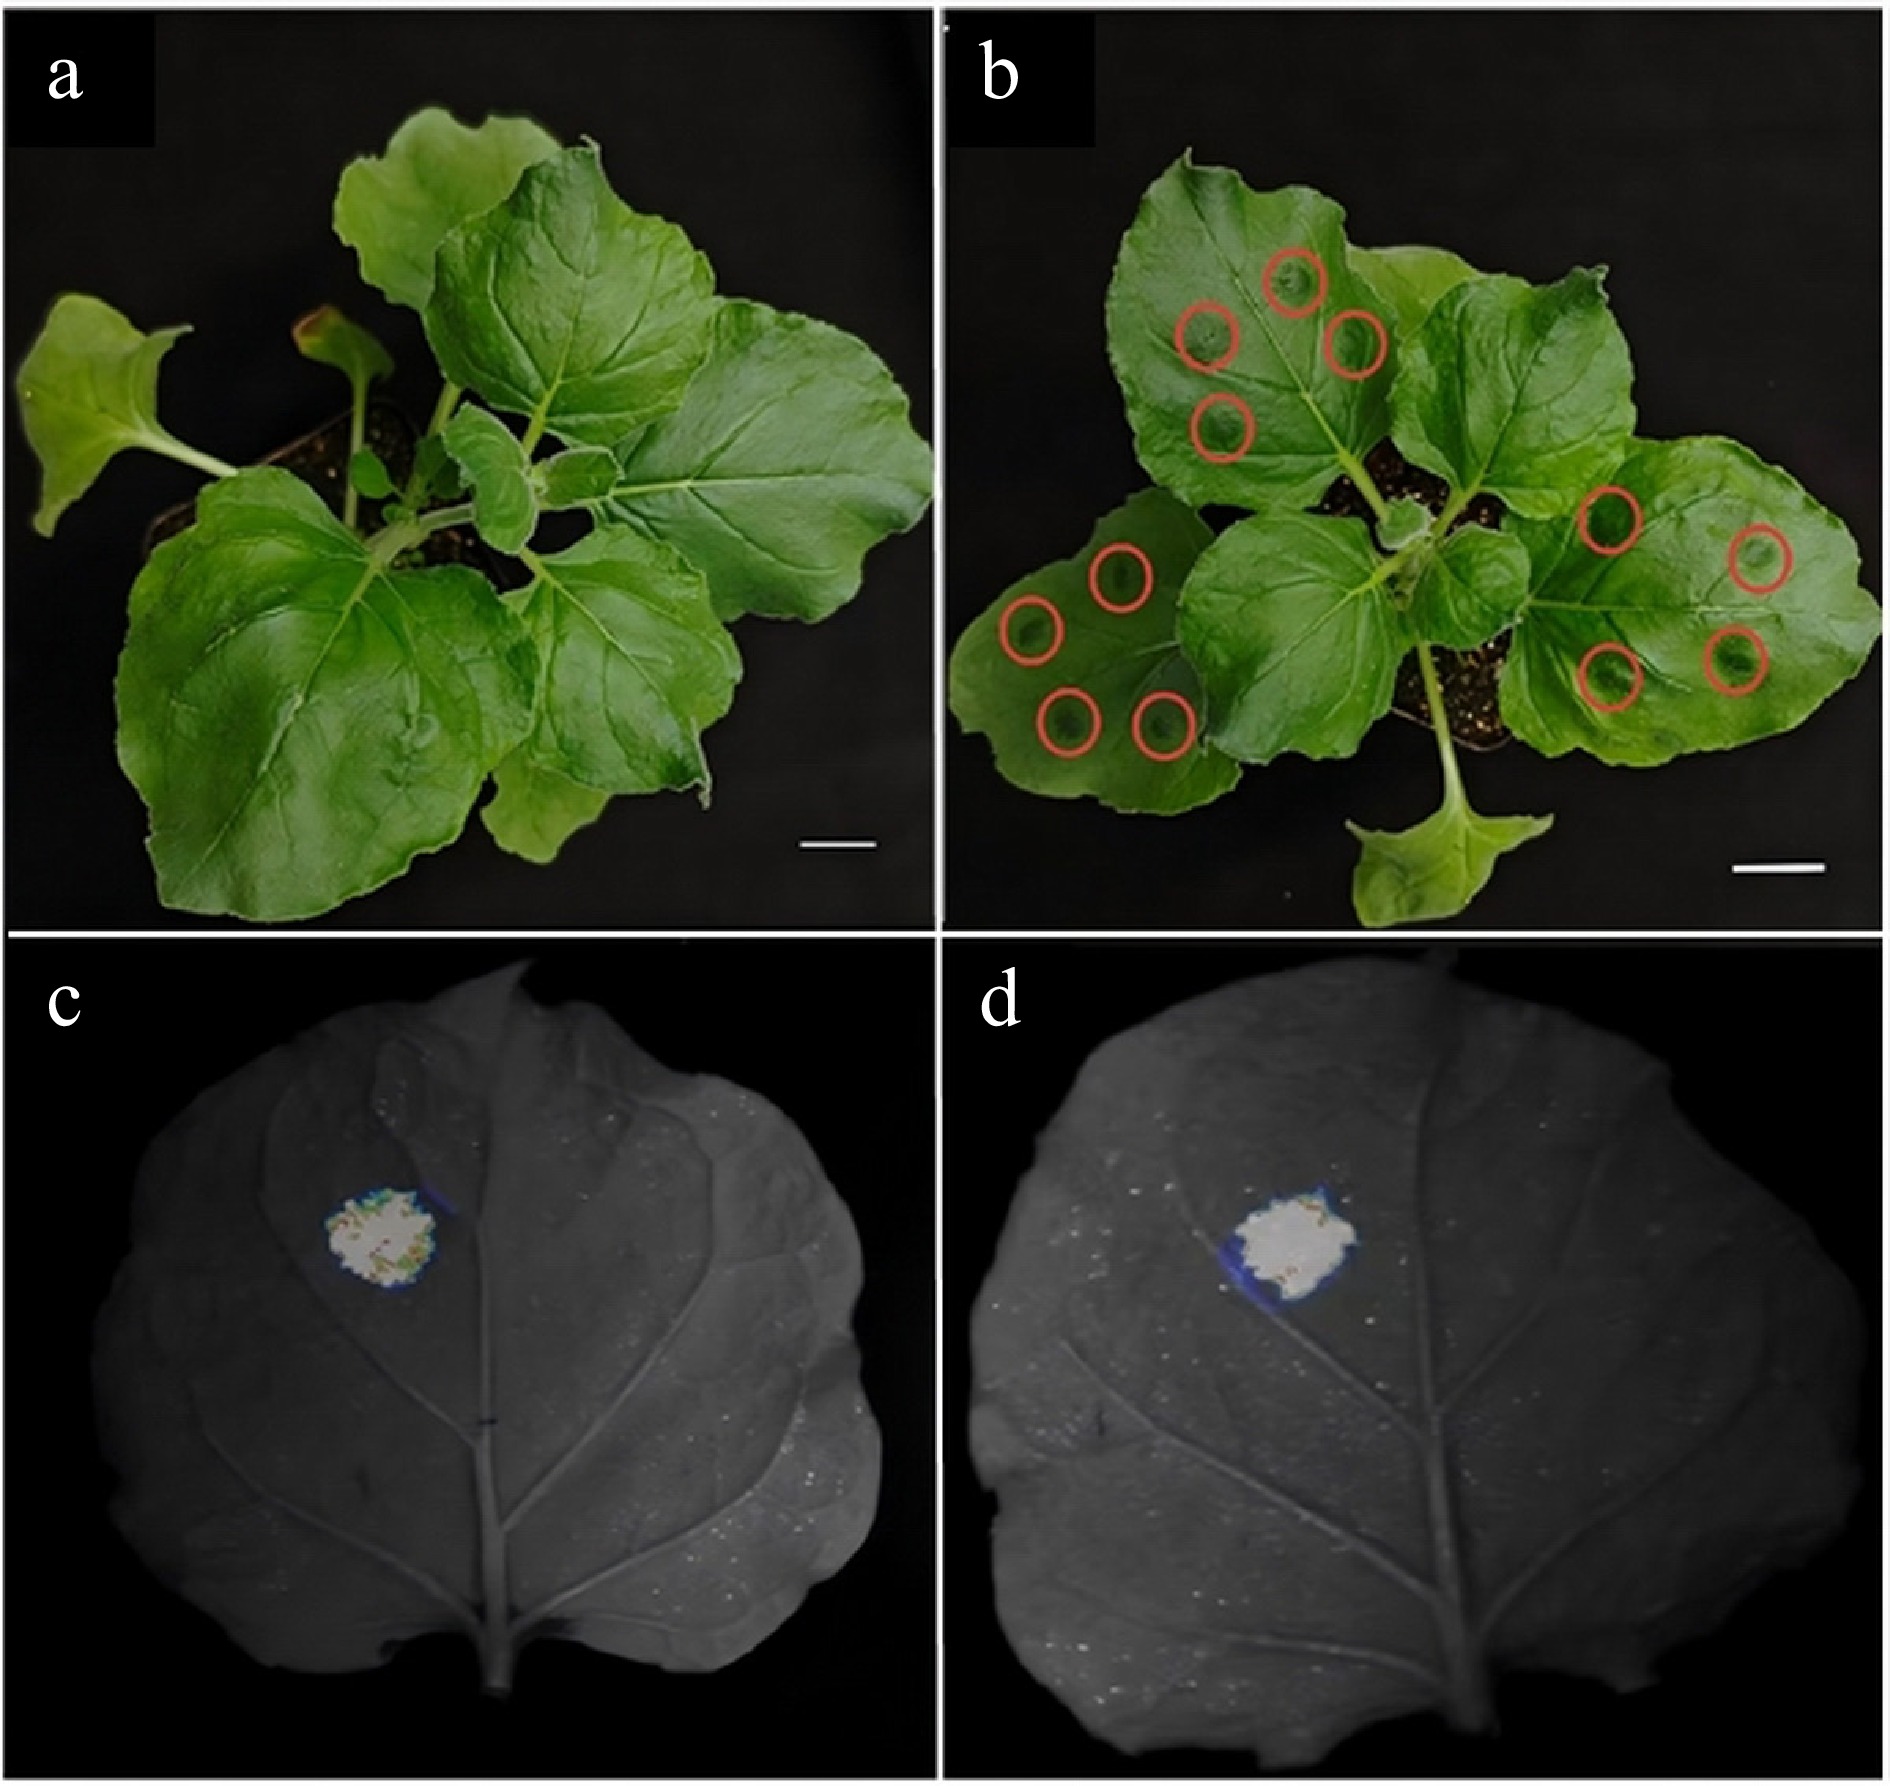
Figure 3.
Protein–protein interaction between EgGRF1/EgGRF7 and EgGIF3 verified by LCI assay in N. benthamiana leaves. (a) Tobacco leaf before injection. (b) Tobacco leaf after injection. (c) Verification of dual-luciferase complementation of EgGRF1 and EgGIF3 genes in tobacco leaves. (d) Verification of dual-luciferase complementation of EgGRF7 and EgGIF3 genes in tobacco leaves. Red circles indicate the injection sites. Scale bar = 1 cm.
Optimization of Agrobacterium-mediated transformation parameters
-
To improve the genetic transformation efficiency of oil palm callus, we systematically evaluated four key parameters: Agrobacterium concentration (OD600), infection duration, acetosyringone (AS) concentration, and co-cultivation time. A factorial experiment with five OD600 values (0.4, 0.5, 0.6, 0.7, 0.8) and four infection durations (20, 30, 40, 50 min) was conducted. GFP-positive calli were observed in 12 out of 20 treatment combinations (Table 1). The highest screening efficiencies were achieved at OD600 = 0.6 with 30 min infection (3.32% ± 0.59%) and at OD600 = 0.5 with 40 min infection (3.45% ± 2.84%). Lower efficiencies (1.12%–2.26%) were observed in other treatments. Notably, no GFP-positive calli were obtained at the highest bacterial concentration (OD600 = 0.8) or the longest infection time (50 min) when combined with certain OD600 values, likely due to callus browning and overgrowth of Agrobacterium.
Table 1. Effects of Agrobacterium concentration and infection time on screening efficiency.
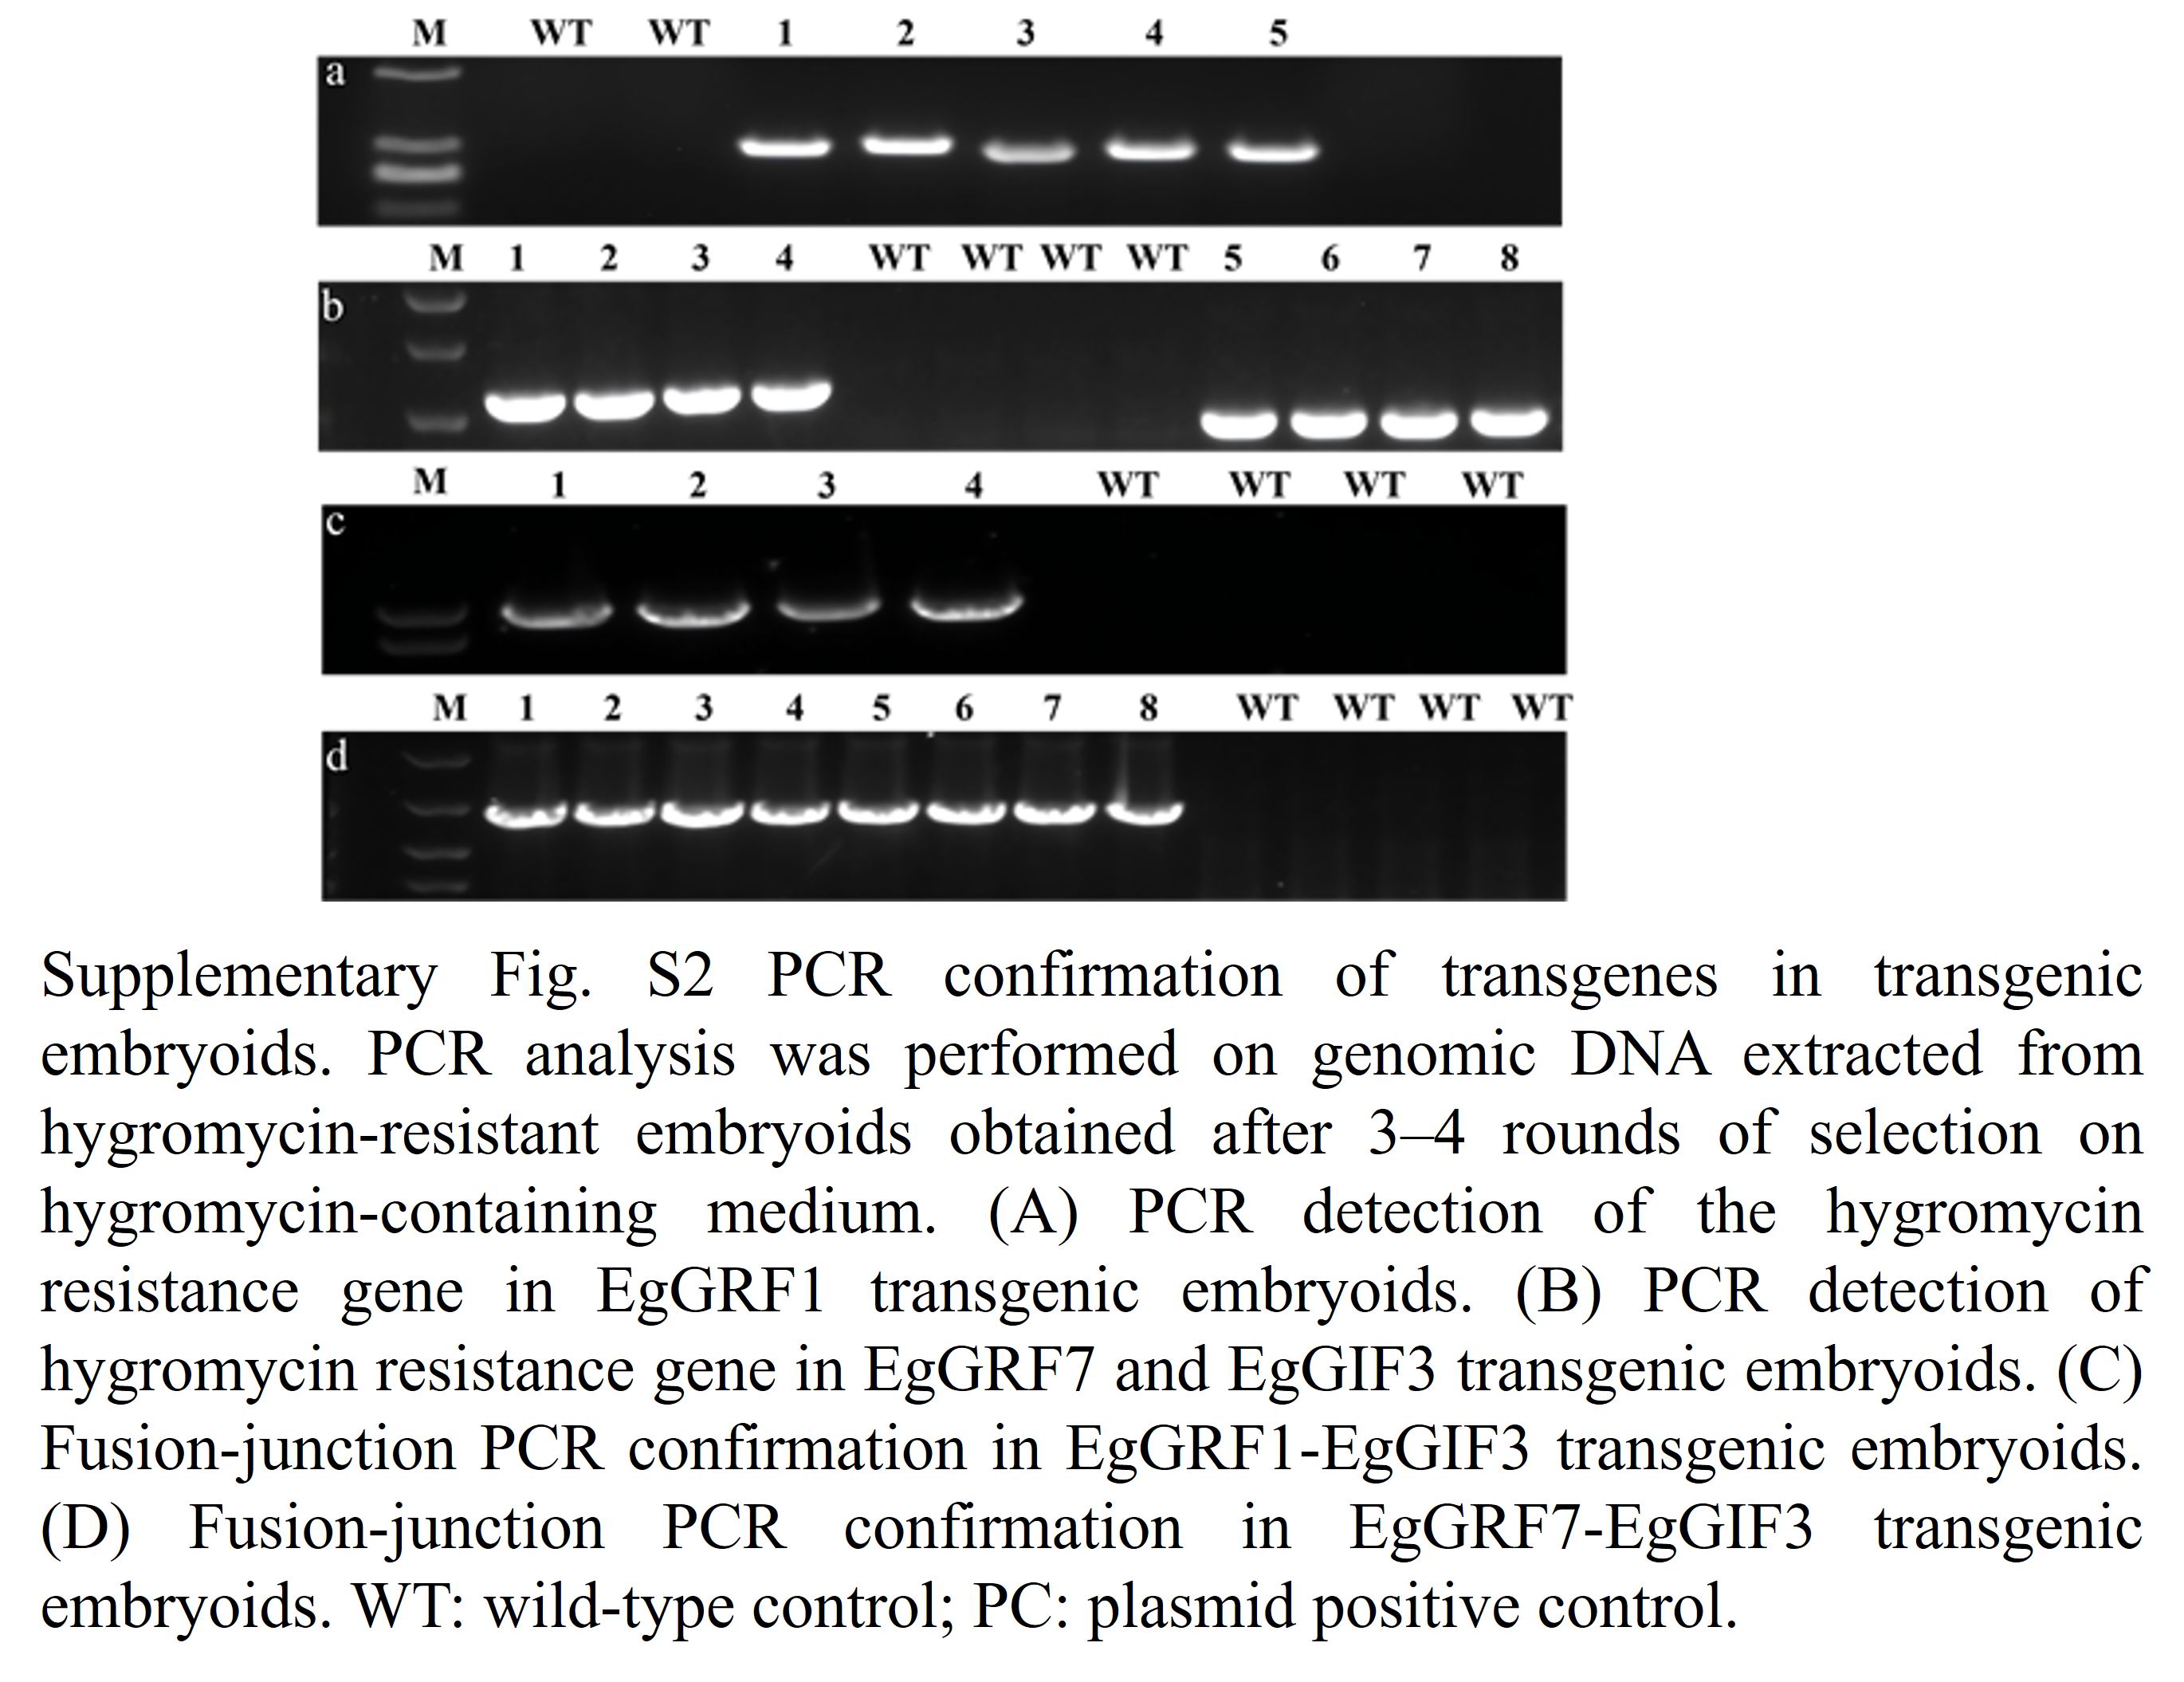
Level Factors OD600 Time (min) Number GFP (%) 1 0.4 40 184 1.12 ± 1.05bc 2 0.6 50 176 0.00 ± 0.00c 3 0.8 50 144 0.00 ± 0.00c 4 0.6 20 167 1.82 ± 0.69bc 5 0.7 20 170 1.17 ± 1.23bc 6 0.5 20 187 0.00 ± 0.00c 7 0.6 30 178 3.32 ± 0.59ab 8 0.4 30 182 2.06 ± 2.01ab 9 0.4 20 163 0.00 ± 0.00c 10 0.7 30 166 0.00 ± 0.00c 11 0.6 40 166 2.21 ± 0.99ab 12 0.7 40 175 0.00 ± 0.00c 13 0.8 20 180 1.51 ± 1.44bc 14 0.8 30 158 1.47 ± 0.57bc 15 0.8 40 159 0.00 ± 0.00c 16 0.5 30 163 1.82 ± 3.15bc 17 0.7 50 169 0.00 ± 0.00c 18 0.5 50 160 1.95 ± 1.99ab 19 0.5 40 174 3.45 ± 2.84ab 20 0.4 50 173 2.26 ± 0.35ab Different letters after the numbers (a, b, c) represent statistical differences between groups; values represent mean ± SD (n = 3). AS concentrations ranging from 50 to 250 μmol/L were tested under optimal infection conditions (OD600 = 0.5, 40 min). The screening efficiency increased with AS concentration up to 200 μmol/L, reaching a maximum of 3.43%, and then declined at 250 μmol/L. Thus, 200 μmol/L AS was selected as the optimal concentration. Co-cultivation durations from 36 to 84 h were evaluated. The screening efficiency increased progressively from 36 to 60 h, peaking at 3.58% at 60 h, and then decreased at longer durations (Fig. 4a, b). Therefore, 60 h was determined as the optimal co-cultivation time. Under the optimized conditions (OD600 = 0.5, infection for 40 min, 200 μmol/L AS, 60 h co-cultivation), the average screening efficiency reached 3.58%. PCR confirmation using hygromycin-specific primers confirmed the presence of the transgene in hygromycin-resistant calli, while no band was detected in wild-type controls (Supplementary Fig. S2).
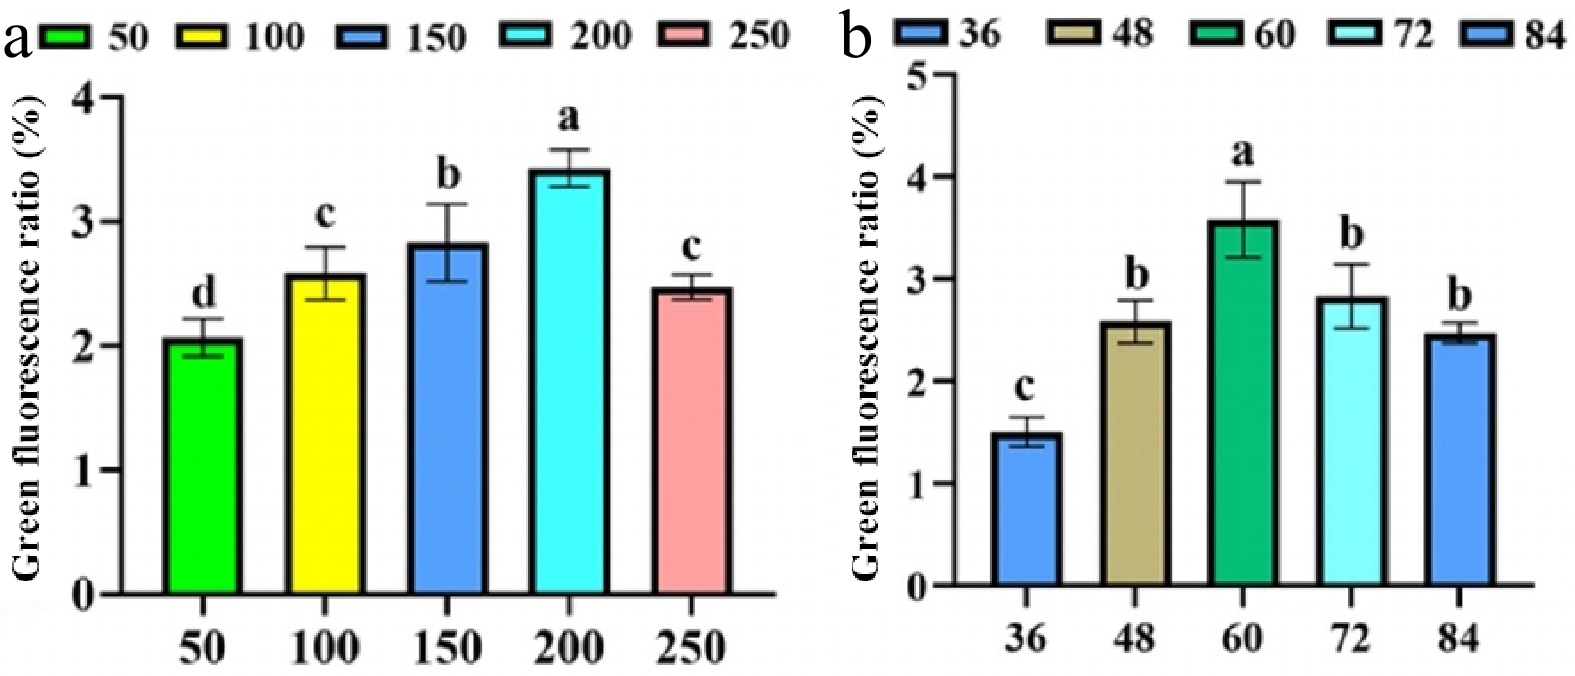
Figure 4.
Effects of (a) acetosyringone (AS) concentration, and (b) co-cultivation duration on Agrobacterium-mediated transformation efficiency of oil palm callus.
Effects of EgGRF and EgGIF overexpression on screening efficiency
-
To evaluate the functional roles of EgGRF1, EgGRF7, EgGIF3, and their co-expression in genetic transformation, we constructed single-gene overexpression vectors (35S:EgGRF1, 35S:EgGRF7, 35S:EgGIF3) and co-expression vectors (35S:EgGRF1-EgGIF3 and 35S:EgGRF7-EgGIF3). These constructs were introduced into oil palm callus using the optimized transformation protocol. After three to four rounds of selection on hygromycin-containing medium (9–12 weeks), transgenic materials at various developmental stages—including embryogenic calli, embryoids, and regenerated shoots—were harvested for molecular analysis. GFP fluorescence was detected in transgenic materials from all transformation treatments at different differentiation stages (Fig. 5a−f), whereas no fluorescence was observed in wild-type controls. PCR analysis was performed on genomic DNA extracted from hygromycin-resistant embryoids, which were the most abundant tissue type obtained after three to four rounds of selection. As shown in Supplementary Fig. S2, the hygromycin resistance gene was successfully amplified from transgenic embryoids across all construct types, while no amplification was detected in wild-type controls.
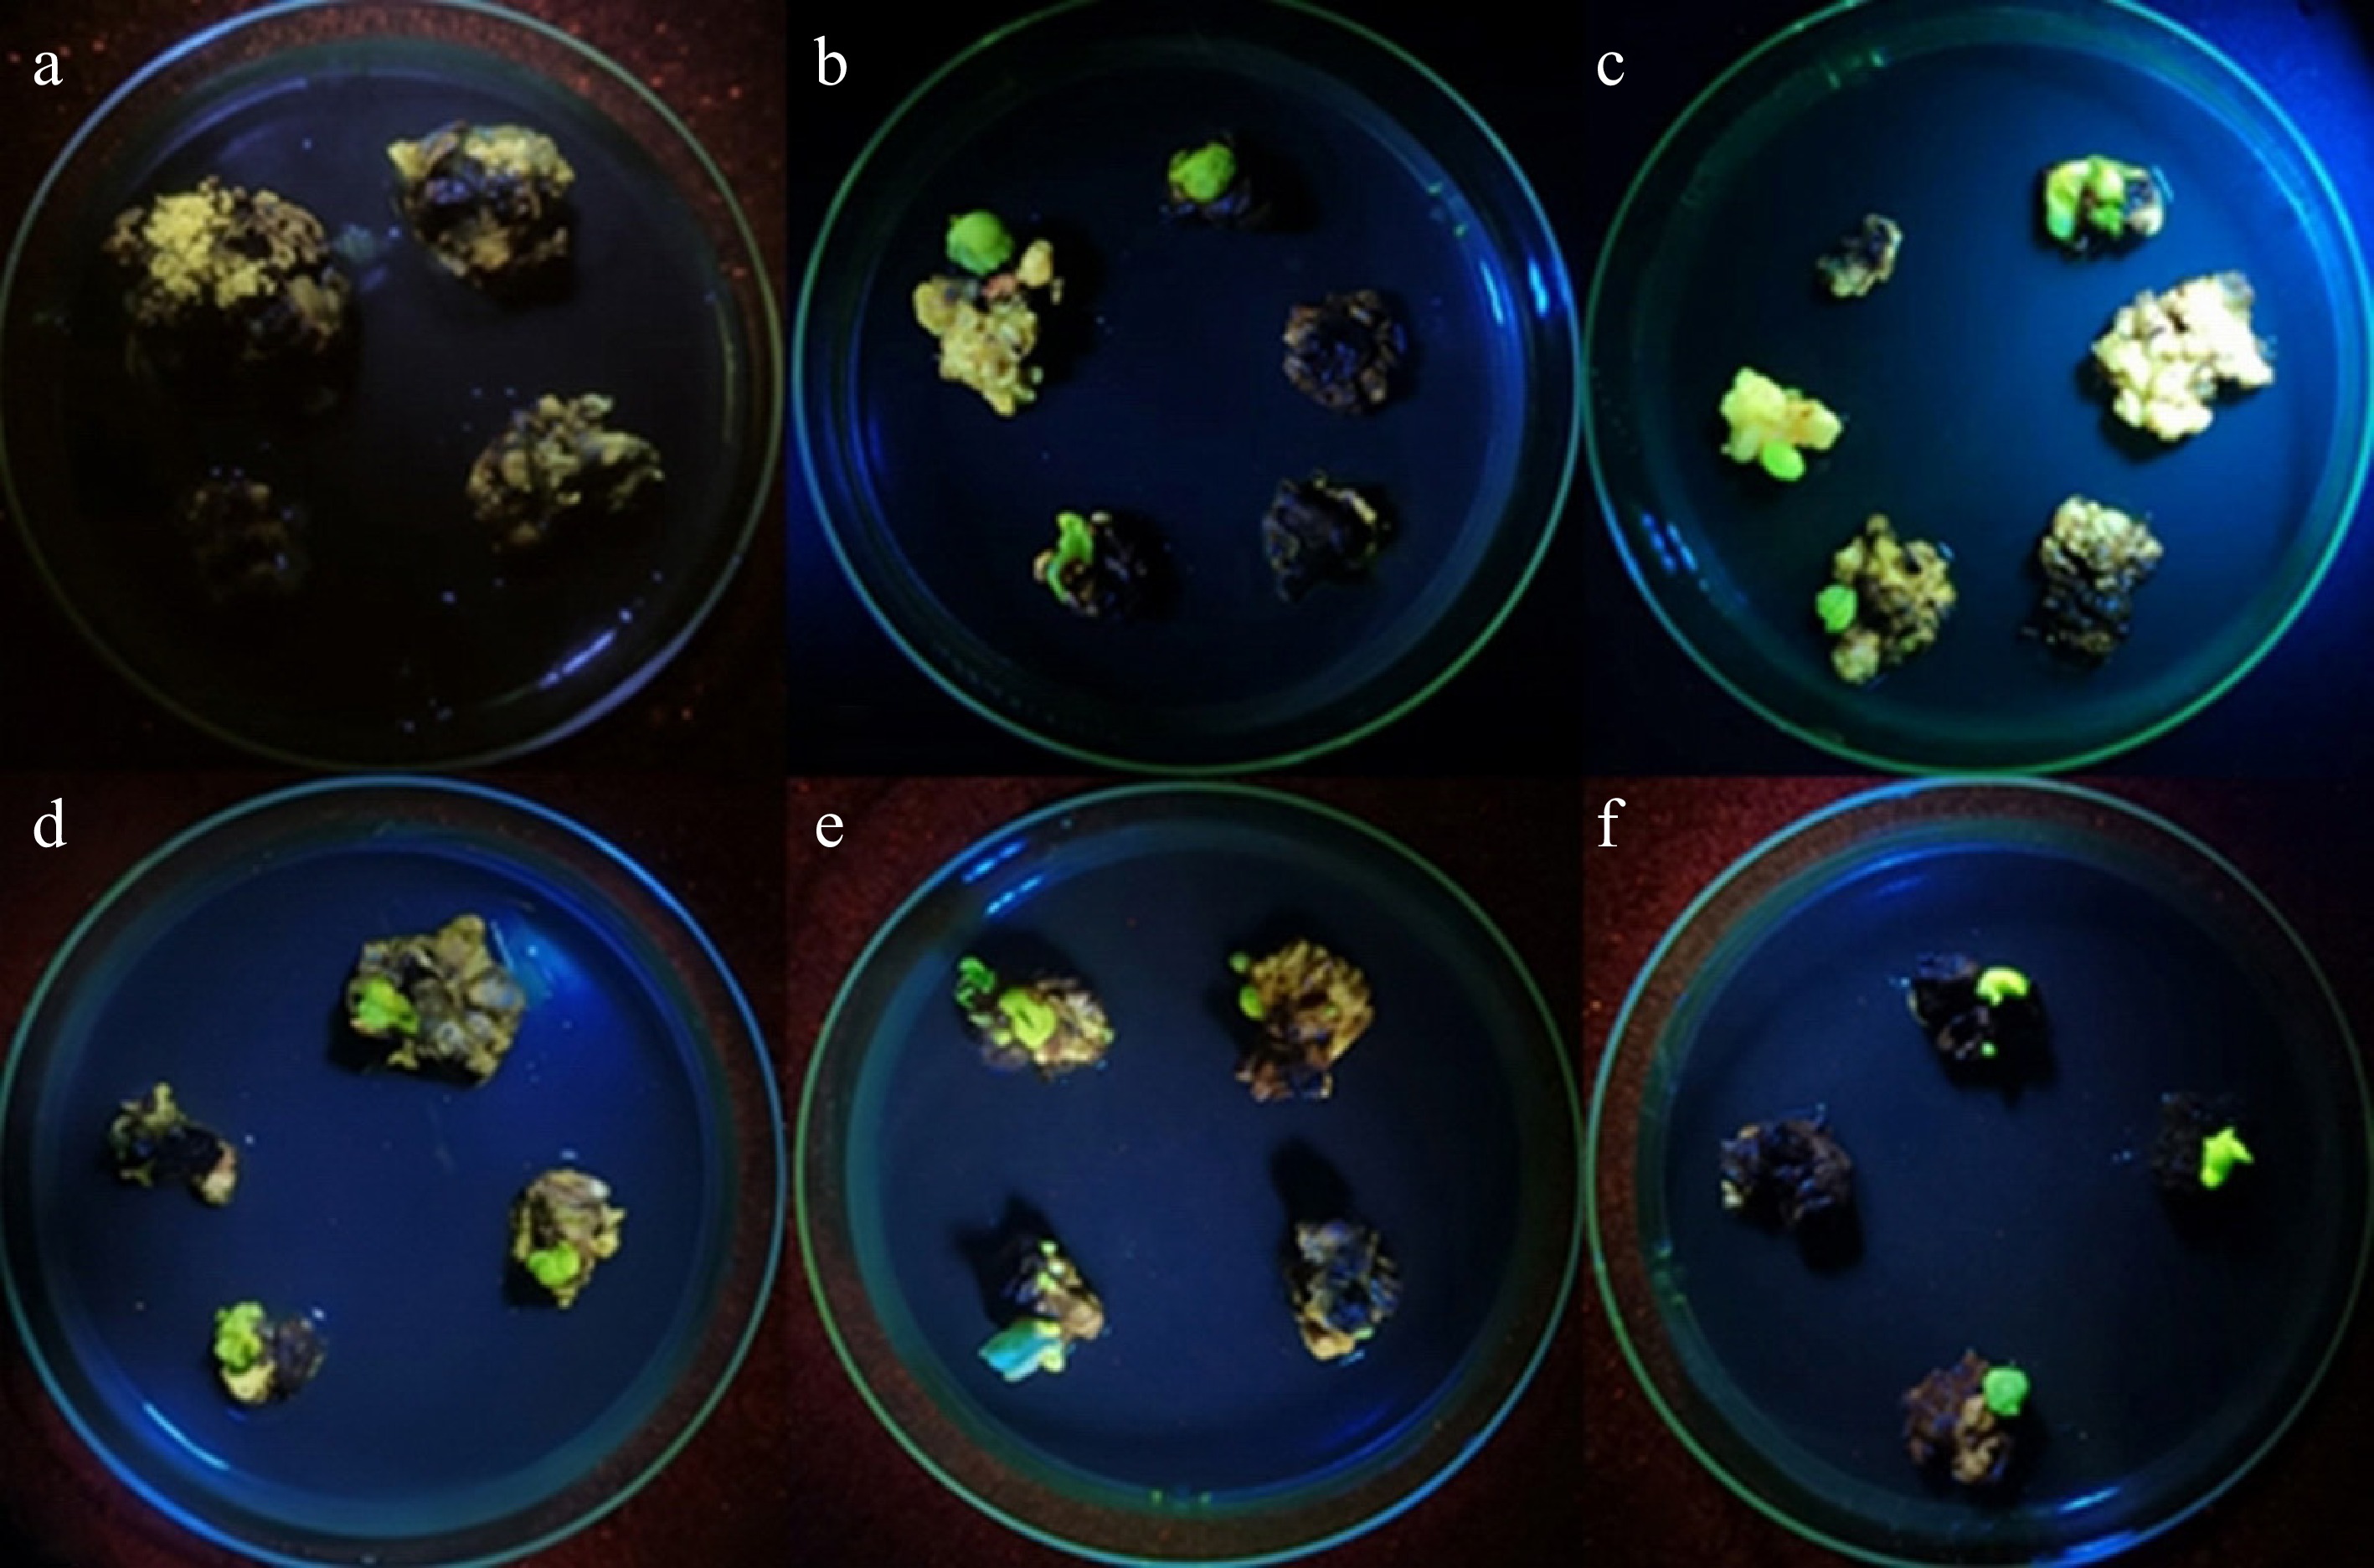
Figure 5.
Visualization and molecular confirmation of transgenic tissues. (a) Wild-type (CK). (b) EgGRF1. (c) EgGRF7. (d) EgGIF3. (e) EgGRF1-GIF3. (f) EgGRF7-GIF3.
RT-qPCR analysis was performed on RNA extracted from transgenic embryoids, which provided the most consistent and abundant material for gene expression analysis. The results revealed that all transgenic embryoids exhibited significantly higher expression levels of the respective target genes compared to wild-type controls. Notably, the EgGRF1-EgGIF3 co-expression calli showed the highest expression levels among all transgenic lines (> 10-fold relative to WT), while EgGRF7-EgGIF3 co-expression calli exhibited even higher expression (> 15-fold). Single-gene transformants showed moderate but significant increases in target gene expression (Fig. 6a−c). The screening efficiency (GFP-positive rate) was calculated for each construct based on the number of GFP-positive embryoids obtained after three to four rounds of selection, as embryoids were the predominant differentiated structures at this stage. The EgGRF1-EgGIF3 co-expression group achieved the highest screening efficiency at 5.32% ± 0.34%, followed by EgGRF1 alone (4.35% ± 0.47%) (Fig. 7a). EgGRF7-EgGIF3 co-expression yielded an efficiency of 4.06% ± 0.22%, while EgGRF7 alone gave 3.46% ± 0.18%. EgGIF3 alone showed the lowest efficiency (2.48% ± 0.50%), which was not significantly different from the empty vector control. Statistical analysis indicated that EgGRF1-EgGIF3 co-expression significantly outperformed all other treatments (p < 0.05), while EgGRF1 alone also showed a significant improvement over the control.
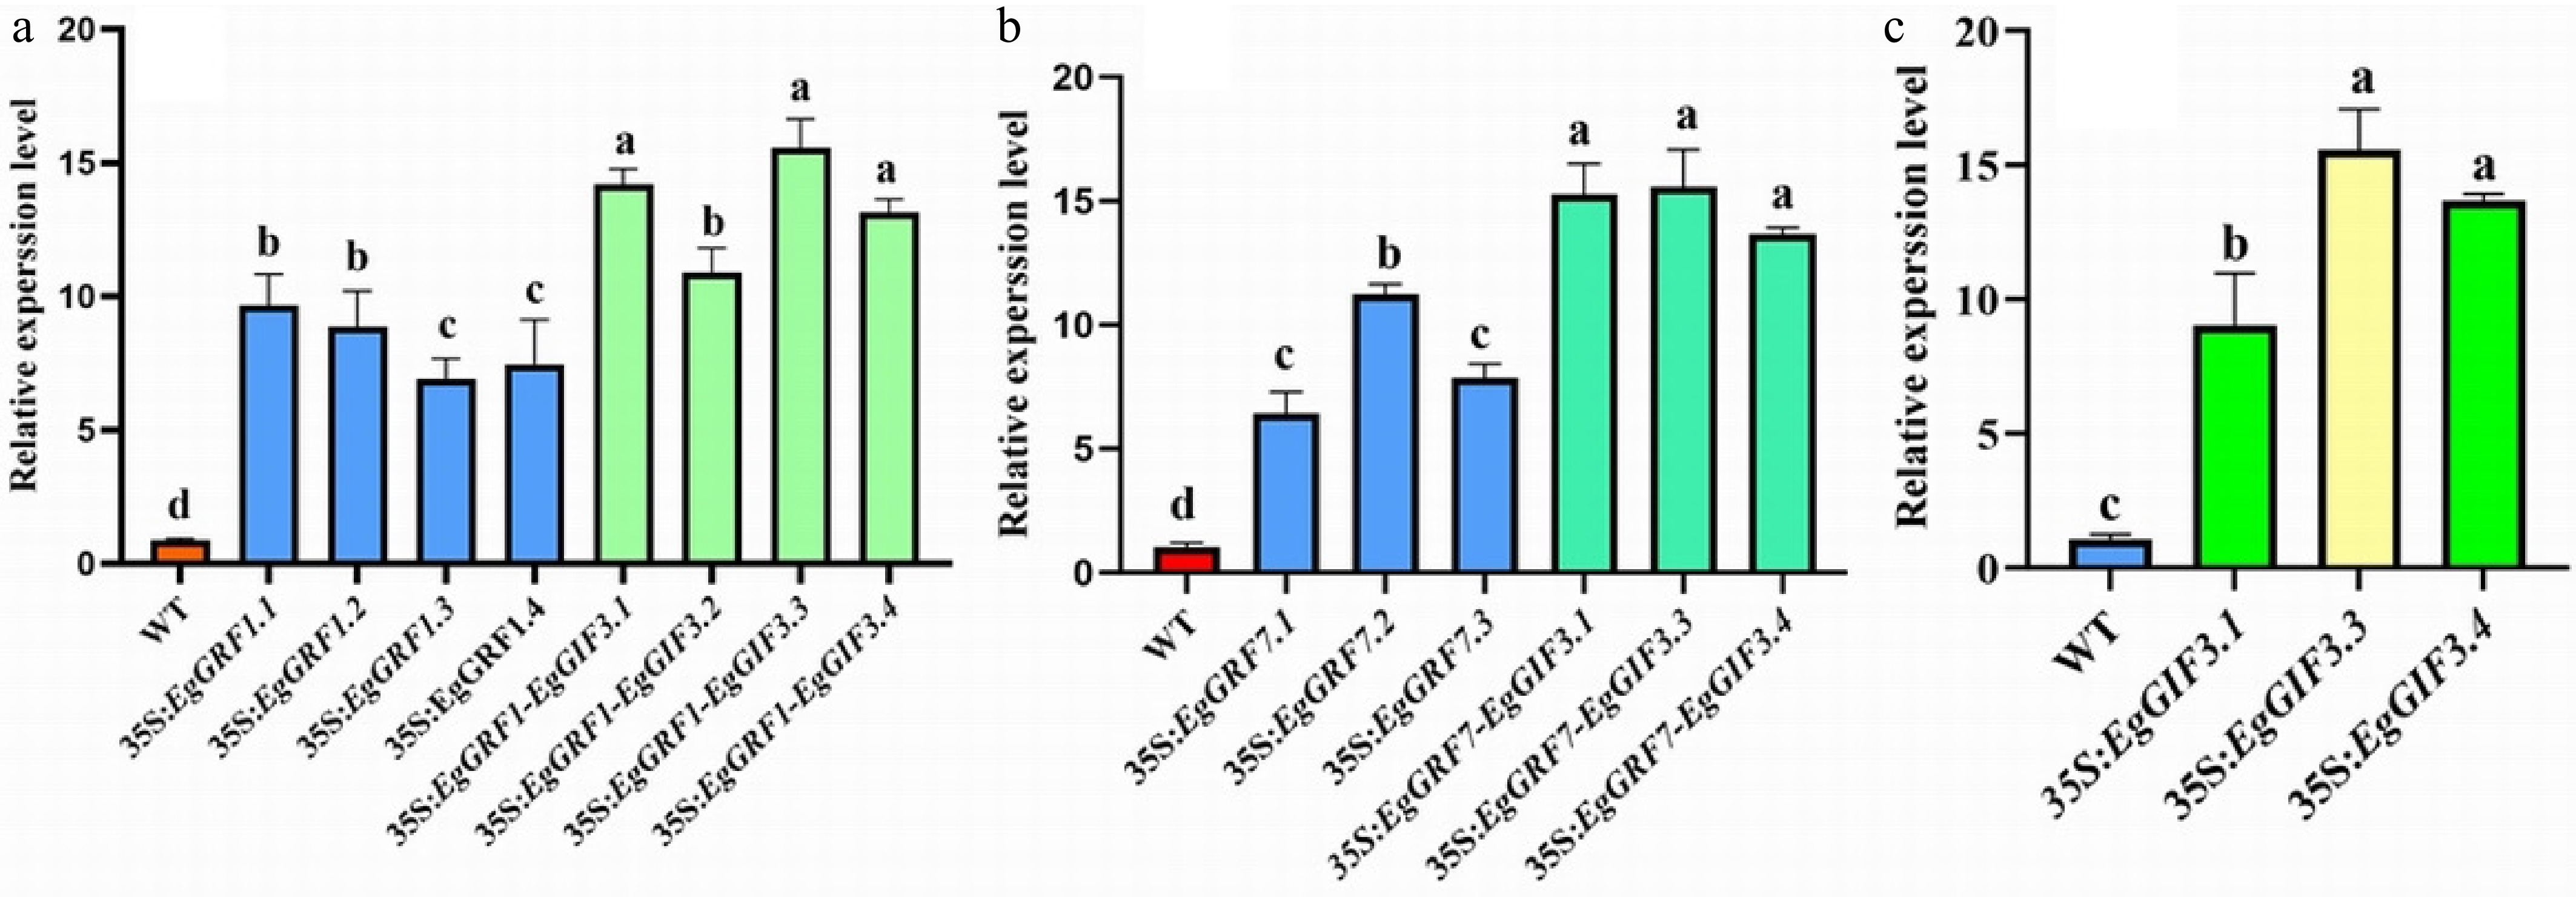
Figure 6.
Relative expression levels of target genes in transgenic embryoids. RT-qPCR analysis was performed on RNA extracted from transgenic embryoids obtained after three to four rounds of selection. (a) Expression levels in embryoids transformed with EgGRF7 and EgGRF1-EgGIF3. (b) Expression levels in embryoids transformed with EgGRF7 and EgGRF7-EgGIF3. (c) Expression levels in embryoids transformed with EgGIF3. Values are mean ± SD (n = 3). Different letters indicate significant differences (p < 0.05).
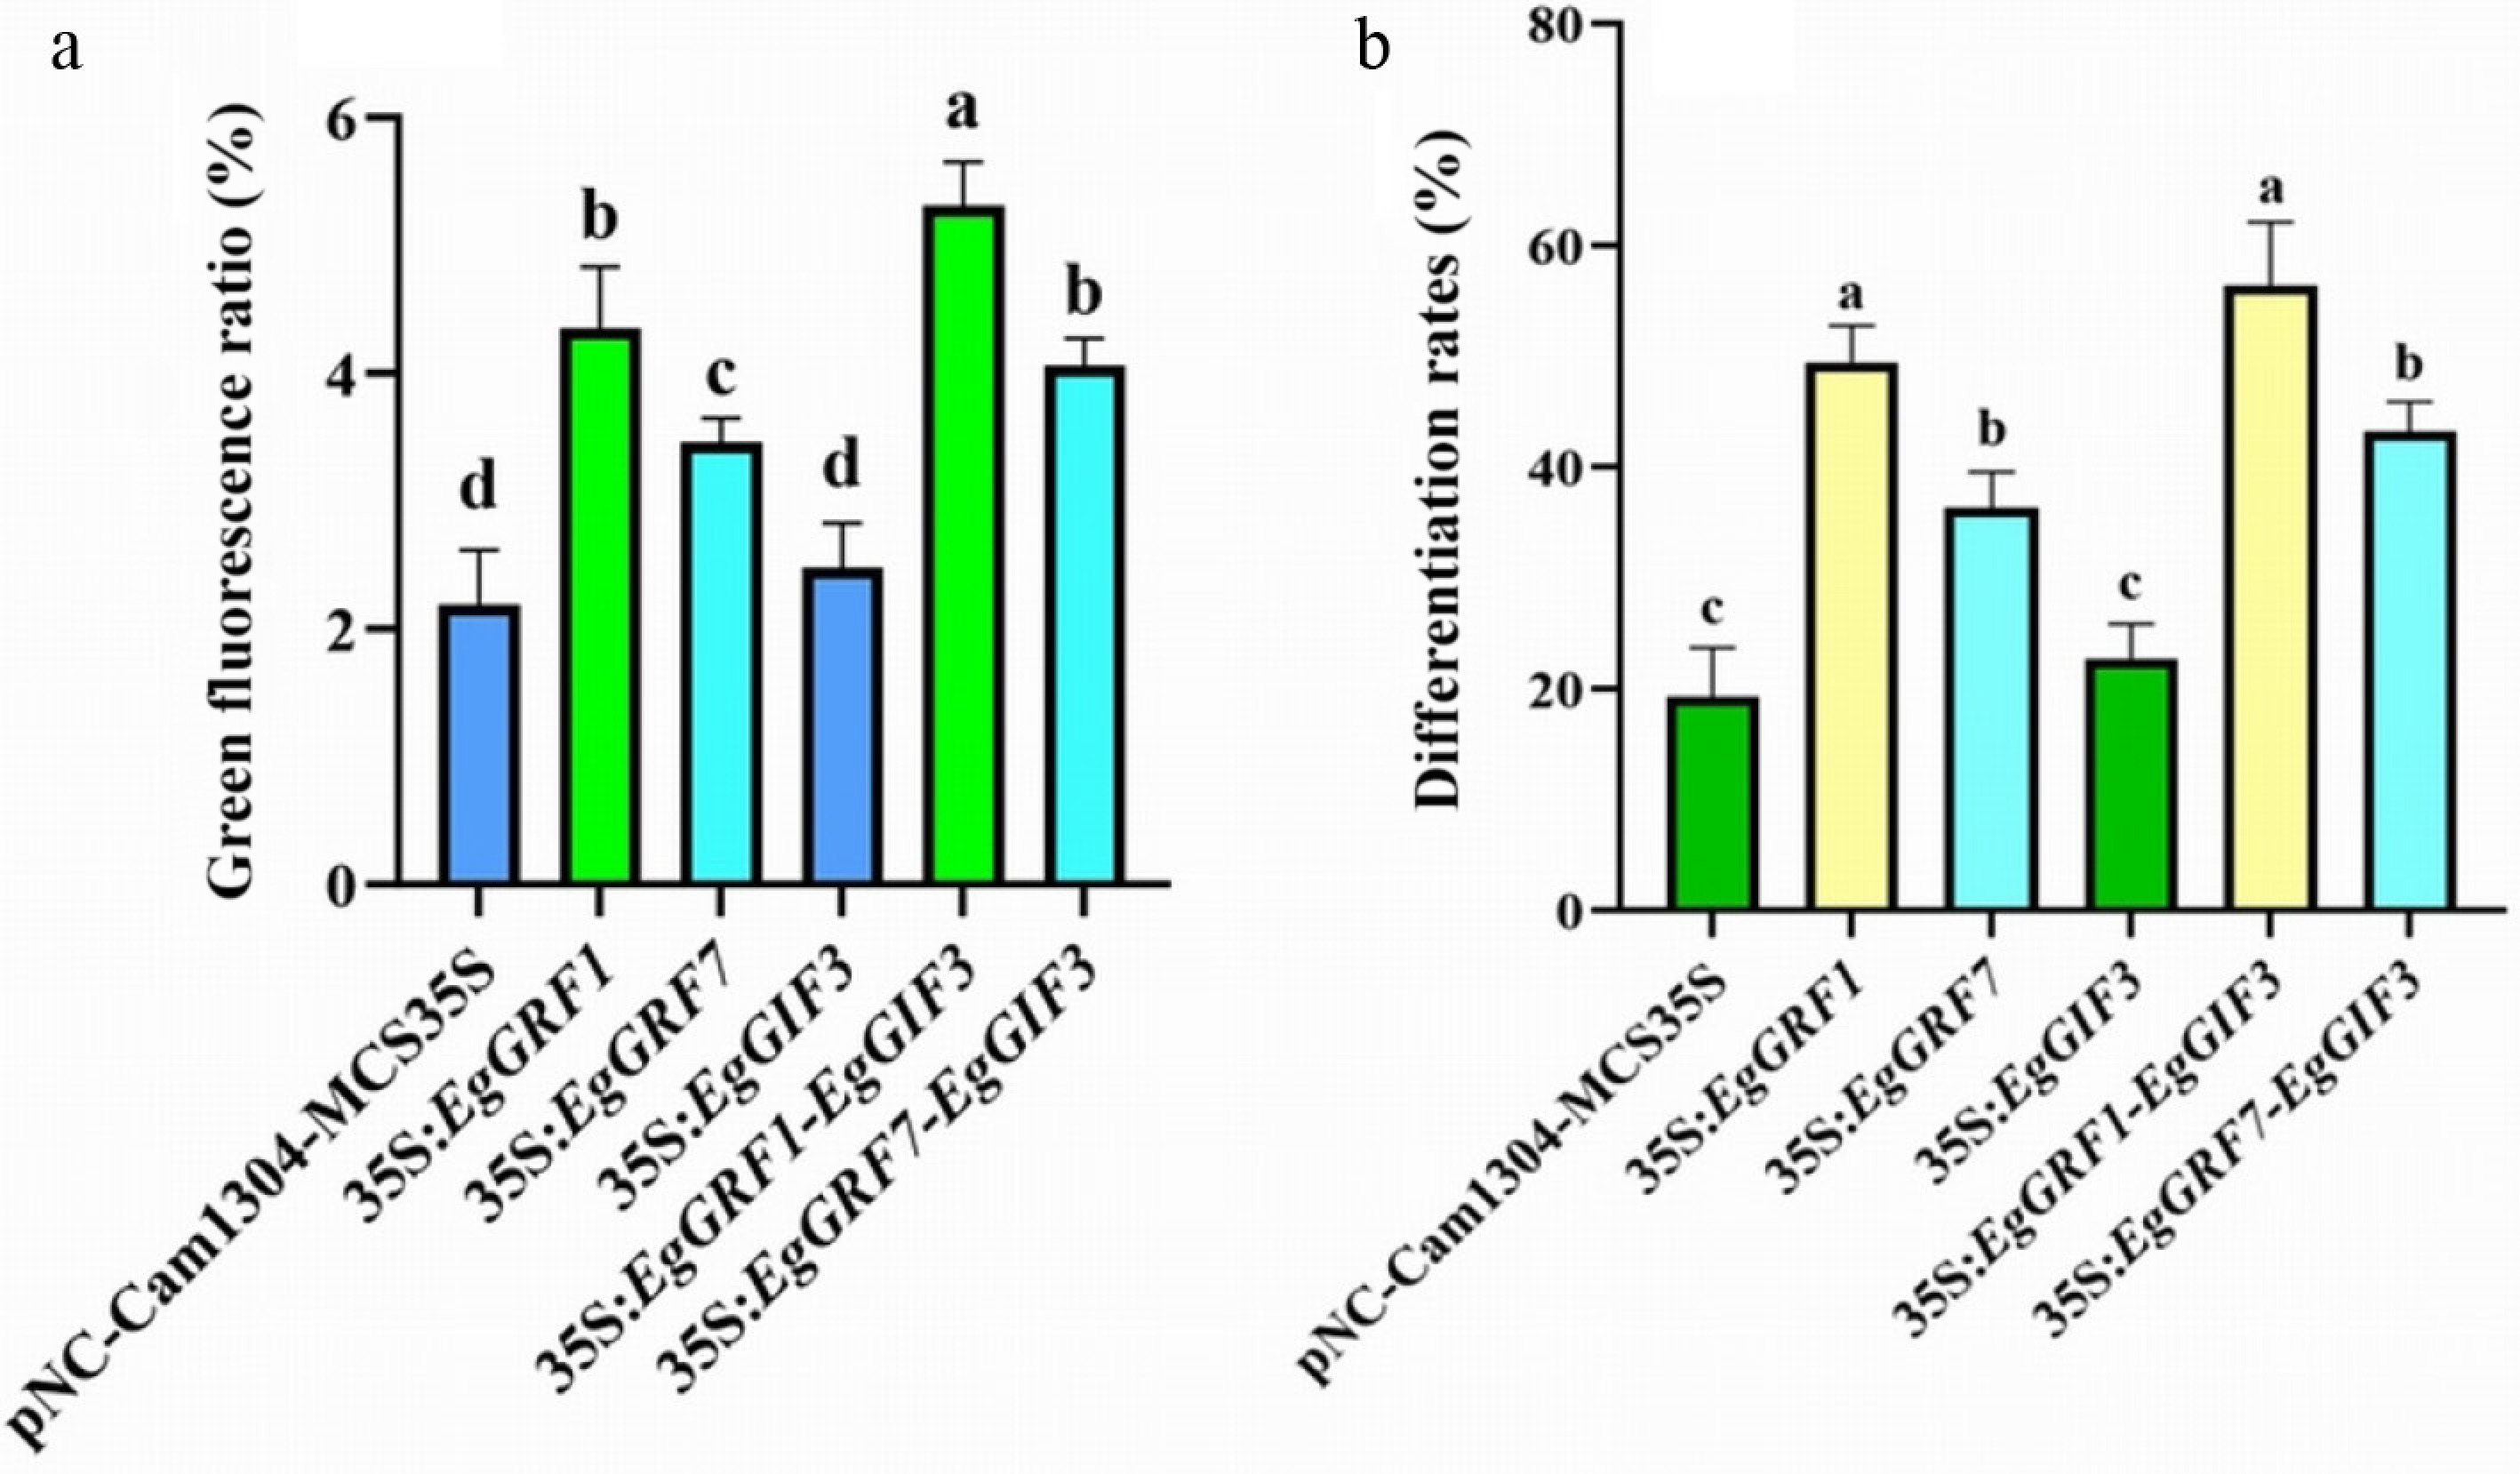
Figure 7.
Effects of EgGRF and EgGIF overexpression on screening efficiency and differentiation. (a) Screening efficiency based on GFP-positive embryoids after three to four rounds of selection. (b) Differentiation rate of transgenic regenerated shoots derived from embryoids. Values are mean ± SD (n = 3). Different letters indicate significant differences (p < 0.05).
Effects of EgGRF and EgGIF overexpression on callus differentiation
-
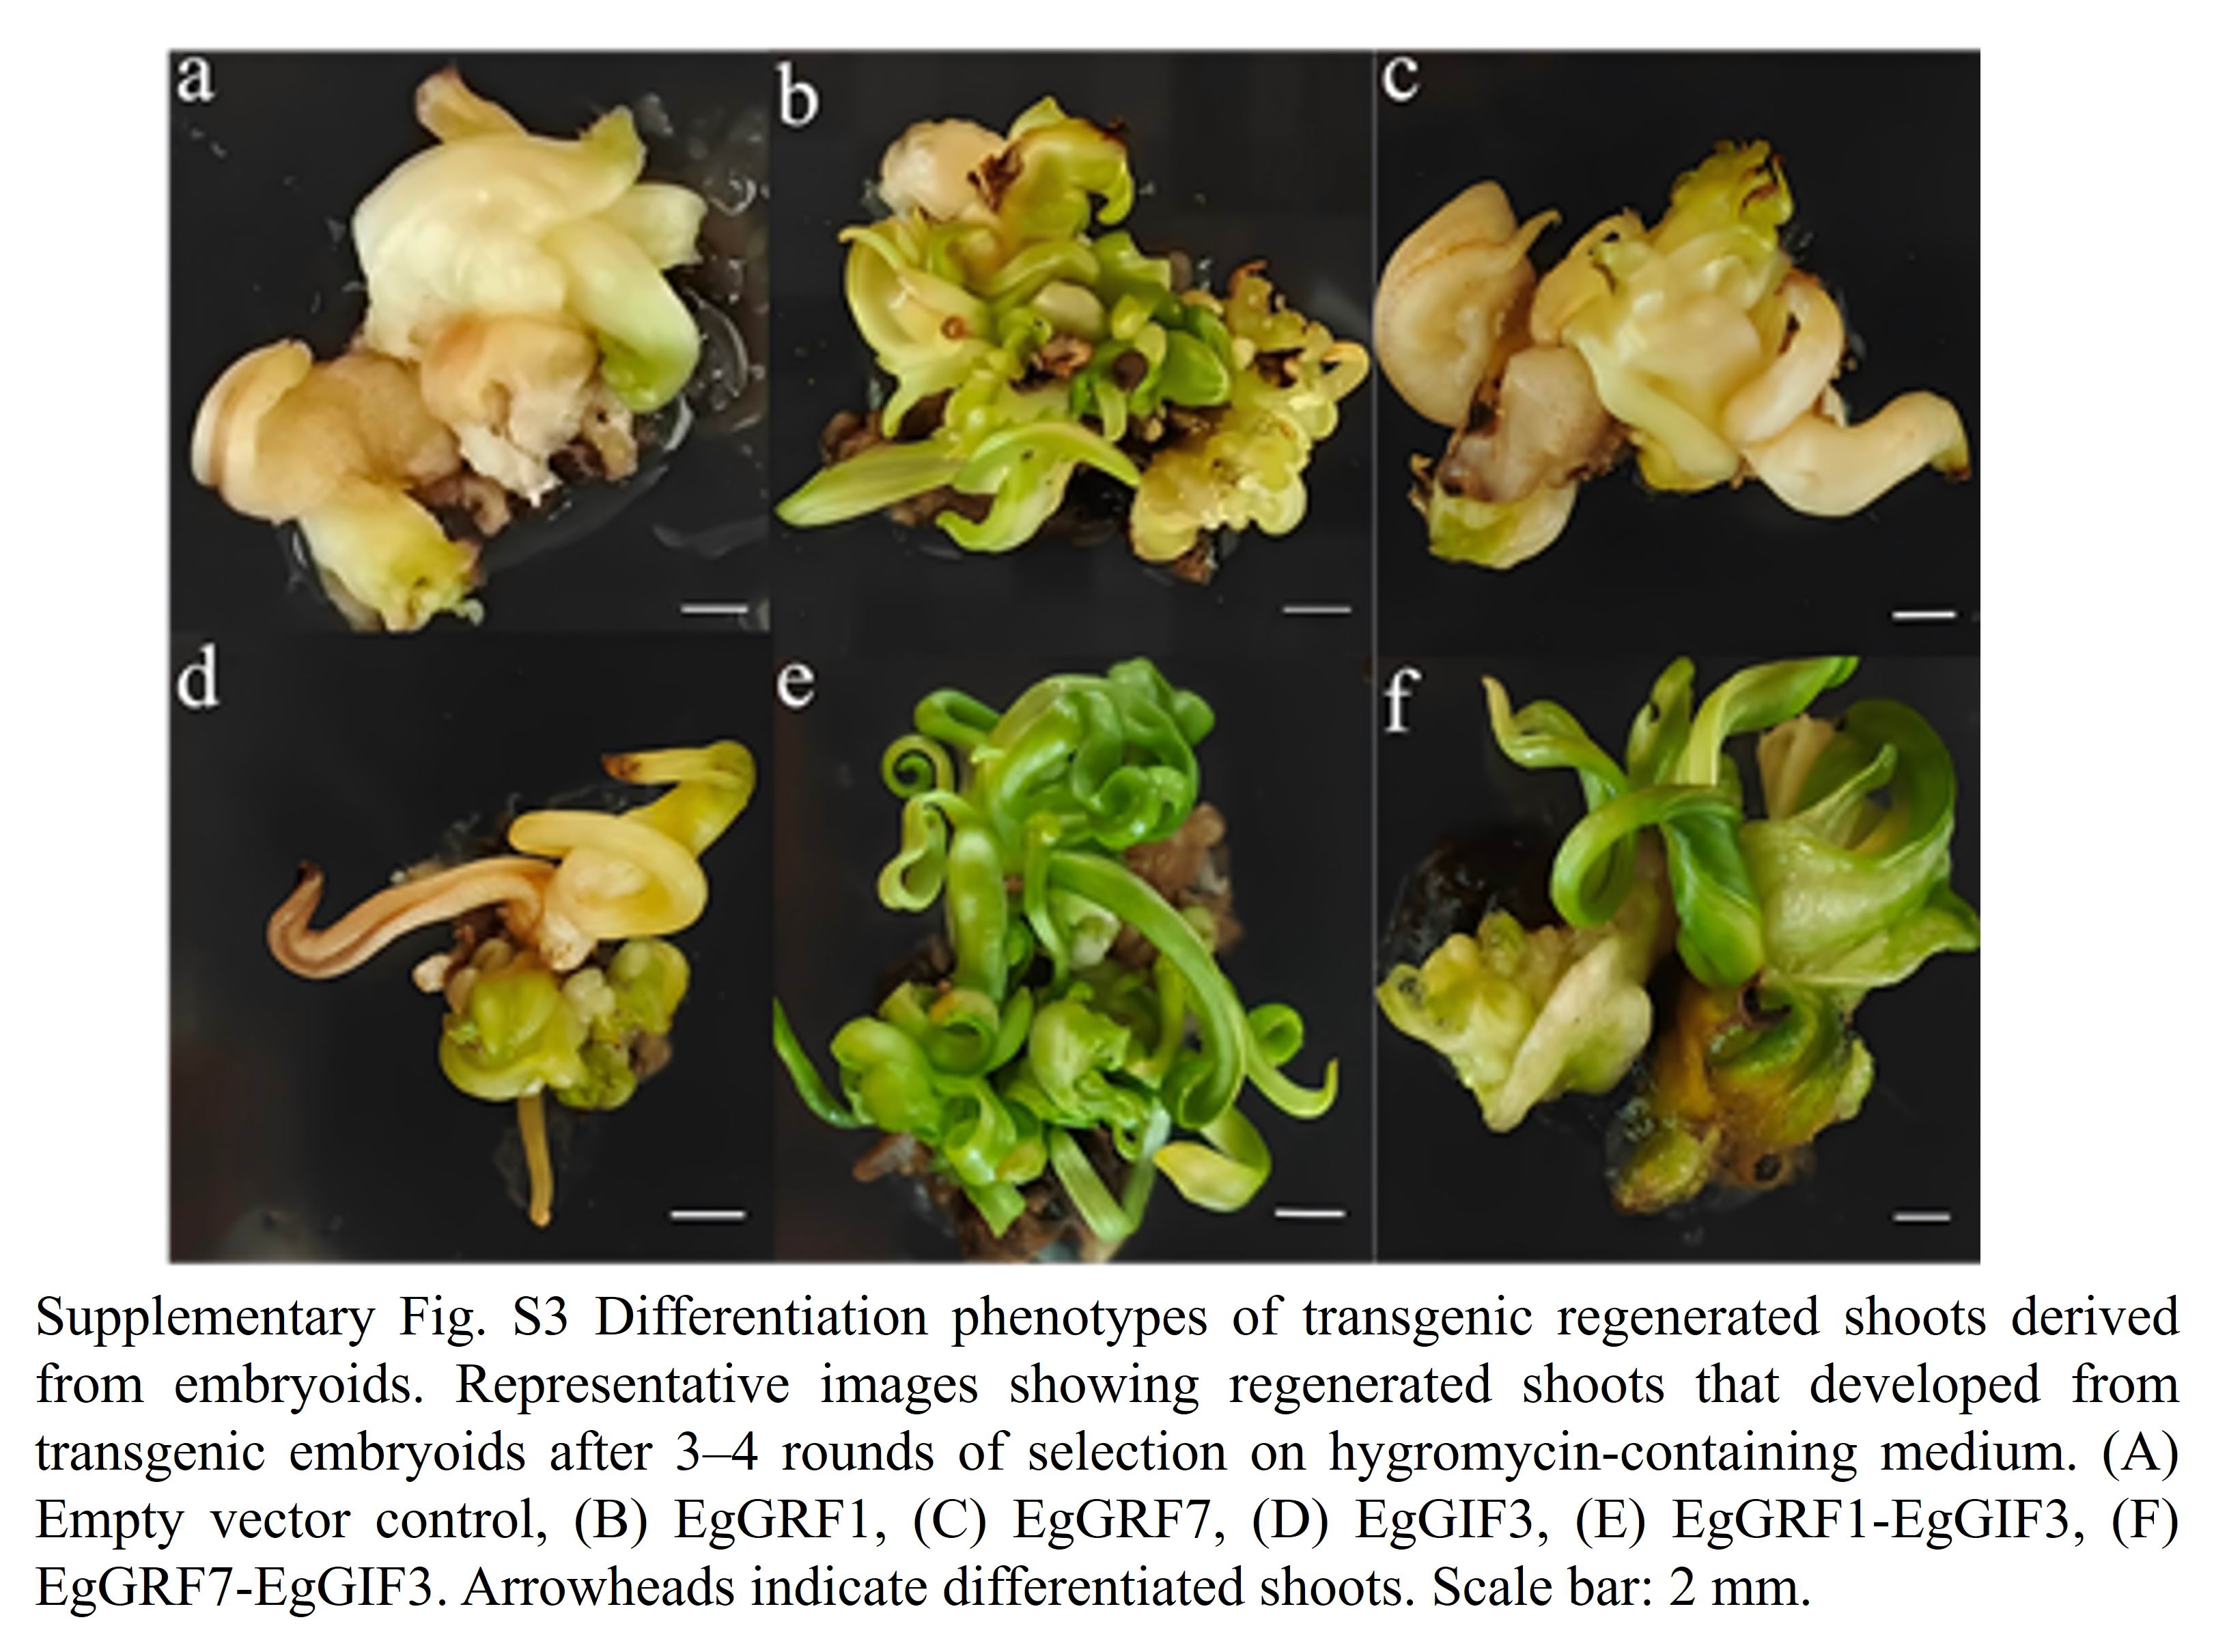
The differentiation capacity of transgenic materials was evaluated after three months of culture on selection medium. The materials scored for differentiation were regenerated shoots that had developed from embryoids (Supplementary Fig. S3), representing a more advanced developmental stage. Representative images showed that newly formed calli were cream-white in color and emerged from the surface of browned original calli. Notably, albino shoots were observed in some transgenic lines, particularly those transformed with EgGRF1, EgGRF1-EgGIF3, and EgGRF7-EgGIF3. After an additional three months under light culture conditions, distinct differentiation phenotypes were observed. Calli transformed with the empty vector, EgGRF7 alone, or EgGIF3 alone produced a small number of large shoots with low density. In contrast, EgGRF1-transformed calli produced multiple clustered shoots with dense, small leaves. The EgGRF1-EgGIF3 co-expression lines exhibited the most vigorous differentiation phenotype, with abundant clustered shoots and well-developed leaves. EgGRF7-EgGIF3 co-expression also promoted differentiation, producing shoots with complete leaves, though to a lesser extent than EgGRF1-EgGIF3 (Supplementary Fig. S3).
Quantitative analysis showed that the differentiation rate of the empty vector control was 19.27%. EgGRF1-EgGIF3 co-expression resulted in the highest differentiation rate (56.39%), followed by EgGRF1 alone (49.46%), with no significant difference between these two groups. EgGRF7-EgGIF3 co-expression gave a differentiation rate of 43.19%, while EgGRF7 alone reached 36.34%. EgGIF3 alone (22.69%) showed no significant improvement over the control (Fig. 7b). These results demonstrate that EgGRF1 plays a key positive role in oil palm callus differentiation, and its synergistic expression with EgGIF3 further enhances differentiation capacity at the embryogenic stage.
-
In this study, 14 EgGRF and four EgGIF genes were identified in the oil palm genome, and we showed that EgGRF1, EgGRF7, and EgGIF3 were significantly upregulated in regenerable callus. Dual-luciferase assays confirmed physical interactions between EgGRF1/EgGRF7 and EgGIF3. We then optimized an Agrobacterium-mediated transformation protocol for oil palm embryogenic callus, achieving a screening efficiency of 3.58% under optimal conditions (OD600 = 0.5, infection for 40 min, 200 μmol/L AS, 60 h co-cultivation). Finally, we demonstrated that EgGRF1-EgGIF3 co-expression significantly increased both screening efficiency (5.32%) and differentiation rate (56.39%), outperforming single-gene transformations. These results establish EgGRF1 as a key positive regulator of oil palm callus differentiation and provide an effective strategy for improving genetic transformation screening and differentiation at the embryogenic stage in this recalcitrant species.
The number of GRF and GIF genes identified in oil palm (14 EgGRFs, four EgGIFs) is comparable to those in Arabidopsis (nine GRFs, three GIFs), rice (12 GRFs, three GIFs), and maize (15 GRFs, four GIFs), indicating that these gene families are highly conserved across angiosperms[12,13,15]. The presence of conserved QLQ/WRC domains in all EgGRF proteins and SSXT domains in all EgGIF proteins further supports functional conservation of the GRF-GIF regulatory module. Our optimized transformation protocol (3.58% screening efficiency) represents a notable improvement over previously reported efficiencies in oil palm, which typically ranged from 0.7% to 2.0%[9,10]. The optimal AS concentration (200 μmol/L) and co-cultivation time (60 h) identified in our study are consistent with protocols for other recalcitrant monocots, which often require stronger Vir gene induction and longer co-cultivation periods compared to herbaceous plants[11]. The finding that EgGRF1-EgGIF3 co-expression enhances screening efficiency and differentiation capacity aligns with the landmark study by Debernardi et al.[22], who showed that GRF-GIF chimeric proteins improve transformation and regeneration efficiency in wheat, rice, and citrus. Notably, while Debernardi et al. demonstrated whole-plant regeneration, our study focuses on the callus/embryogenic stage as a platform for rapid functional gene validation in oil palm. Notably, EgGRF1 alone significantly improved differentiation rate (49.46%), whereas EgGIF3 alone showed no effect, consistent with the role of GIFs as co-activators that require GRF partners to function[19].
Taken together, to our knowledge, this is the first comprehensive analysis of GRF and GIF genes in oil palm and demonstrates the practical application of GRF-GIF co-expression to enhance genetic transformation in this crop. PCR and GFP analyses confirmed transgene integration and expression in transgenic materials at multiple stages of in vitro development, including embryogenic calli, embryoids, and regenerated shoots. These data demonstrate that the EgGRF1-EgGIF3 co-expression module promotes not only screening efficiency at the callus stage but also differentiation capacity leading to early shoot formation. However, it should be clearly stated that the production of complete, soil-grown transgenic plants was not pursued in this study, as the primary objective was to establish an efficient transformation platform at the callus/embryogenic stage for rapid functional gene validation in oil palm—a species in which stable transformation and regeneration remain notoriously time-consuming (typically requiring approximately 1 year from callus to plantlet). Whether the improved efficiencies observed at the callus/embryogenic stage translate to full plant regeneration remains an important question for future investigation.
-
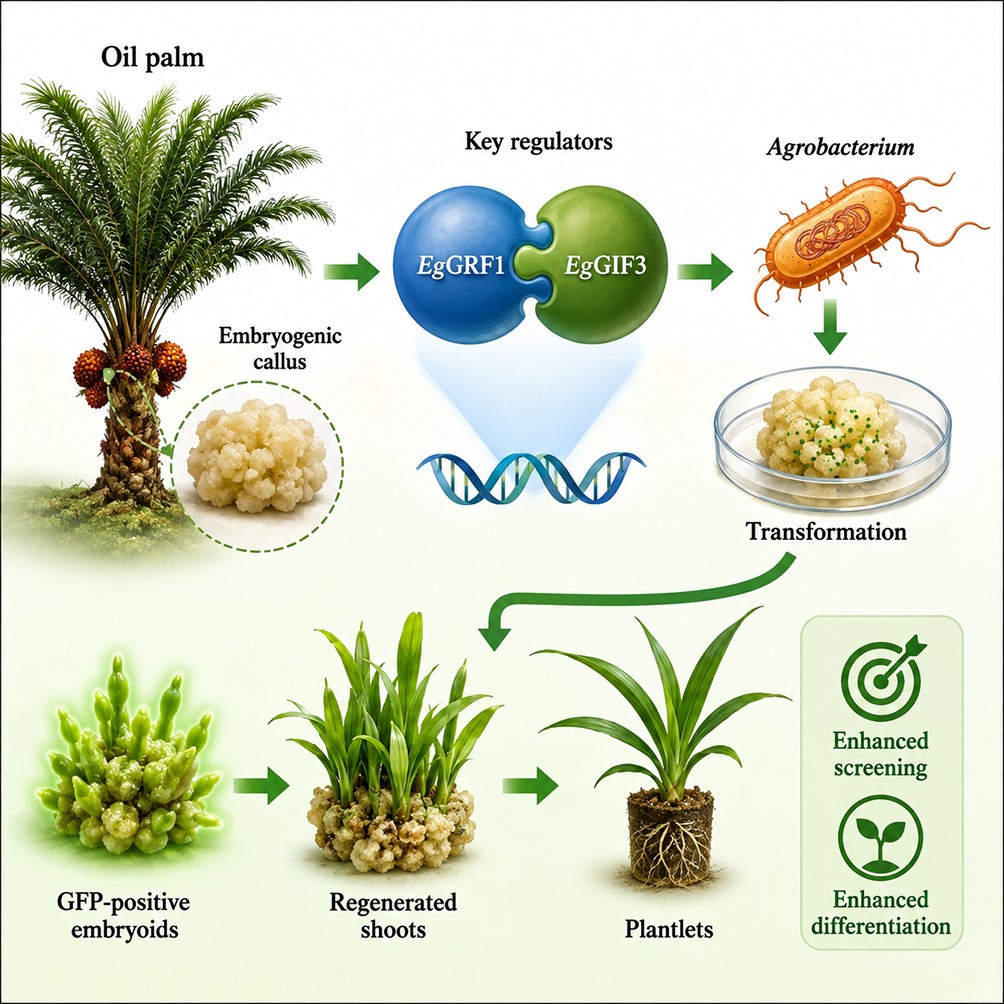
During the preparation of this work, the authors used ChatGPT (GPT-5.5, OpenAI; Date of Use: August 2026) and the OpenAI Image Generation tool to assist in the conceptual design and preparation of the Graphical Abstract. The AI tools were used solely to generate an initial conceptual illustration based on the authors' original research. The authors reviewed, revised, and manually edited the AI-generated content to ensure its scientific accuracy and consistency with the manuscript. The authors take full responsibility for the integrity, originality, and accuracy of the final manuscript and figures. No AI tool is credited as an author.
-
The authors confirm their contributions to the paper as follows: supervision, resources, funding acquisition: Zou J, Li D; data collection: Luo C, Zhang T, Yuan F; analysis and interpretation of results: Luo C, Ouyang C, Zou J; draft manuscript preparation: Luo C, Li D. All authors reviewed the results and approved the final version of the manuscript.
-
The datasets generated during and/or analyzed during the current study are not publicly available because they are being used in ongoing research but are available from the corresponding author on reasonable request.
-
The authors declare that they have no conflict of interest.
-
accompanies this paper online at: https://doi.org/10.48130/tp-0026-0032.
-
Received 20 April 2026; Accepted 22 July 2026; Published online 18 September 2026
- Supplementary Table S1 Physicochemical properties analysis of the EgGRF gene family in oil palm.
- Supplementary Fig. S1 Chromosomal localization and synteny analysis of EgGRF and EgGIF gene family members in oil palm.
- Supplementary Fig. S2 PCR confirmation of transgenes in transgenic materials at different developmental stages.
- Supplementary Fig. S3 Differentiation of transgenic tissues.
- Copyright: © 2026 by the author(s). Published by Maximum Academic Press on behalf of Hainan University. This article is an open access article distributed under Creative Commons Attribution License (CC BY 4.0), visit https://creativecommons.org/licenses/by/4.0/.
-
About this article
Cite this article
Luo C, Zhang T, Yuan F, Ouyang C, Zou J, et al. 2026. EgGRF1-EgGIF3 co-expression enhances transformation and screening efficiency in Agrobacterium-mediated transformation of oil palm. Tropical Plants 5: e032 doi: 10.48130/tp-0026-0032 

EgGRF1-EgGIF3 co-expression enhances transformation and screening efficiency in Agrobacterium-mediated transformation of oil palm
- Received: 20 April 2026
- Revised: 14 July 2026
- Accepted: 22 July 2026
- Published online: 18 September 2026
Abstract: Oil palm (Elaeis guineensis Jacq.) is a tropical woody oil crop with high economic value, but its low genetic transformation efficiency hinders molecular breeding. Growth-regulating factors (GRFs) and GRF-interacting factors (GIFs) play key roles in plant regeneration, yet their functions in oil palm remain unexplored. Here, we identified 14 EgGRF and 4 EgGIF genes via genome-wide analysis. Transcriptome and RT-qPCR showed that EgGRF1, EgGRF7, and EgGIF3 were significantly upregulated in regenerable tissues, and dual-luciferase assays confirmed protein interactions between EgGRF1/EgGRF7 and EgGIF3. We then optimized Agrobacterium-mediated transformation parameters, achieving a screening efficiency of 3.58% under optimal conditions (OD600 = 0.5, infection for 40 min, 200 μmol/L acetosyringone, 60 h co-cultivation). Functional evaluation revealed that EgGRF1-EgGIF3 co-expression significantly increased both screening efficiency (5.32% ± 0.34%) and differentiation rate (56.39%), outperforming single-gene transformations. EgGRF1 alone also markedly improved differentiation (49.46%). Collectively, these results demonstrate that EgGRF1 is a key positive regulator of oil palm callus differentiation, and its synergistic expression with EgGIF3 further enhances screening efficiency and differentiation capacity at the embryogenic stage, providing an optimized protocol and candidate genes for oil palm genetic improvement.
-
Key words:
- Oil palm /
- GRF-GIF co-expression /
- Callus regeneration /
- Screening efficiency /
- Growth-regulating factor