










-
Abiotic stresses—drought, salinity, extreme temperatures, osmotic imbalance, and oxidative overload—are the primary drivers of yield losses in global agriculture, accounting for estimated annual losses exceeding USD 99 billion and affecting more than 50% of cultivated land[1]. Climate projections indicate that the frequency and severity of such events will intensify over the coming decades, placing strong pressure on crop productivity and food security[1,2]. A robust mechanistic understanding of how plants sense and respond to abiotic stress is therefore not merely an academic exercise but a prerequisite for informed crop improvement strategies.
Plant immunity has classically been conceptualized through the lens of pathogen defense, organized around two tiers: pattern-triggered immunity (PTI), initiated by surface receptors recognizing conserved pathogen-associated molecular patterns (PAMPs), and effector-triggered immunity (ETI), mediated by intracellular NLR (nucleotide-binding leucine-rich repeat) receptors that detect pathogen effectors[3,4]. Systemic long-term resistance is further classified as systemic acquired resistance (SAR), predominantly mediated by salicylic acid (SA), and induced systemic resistance (ISR), driven by jasmonate and ethylene (JA/ET) signaling[4]. Although these frameworks elegantly describe plant–pathogen interactions, they fundamentally fail to capture the mechanistic complexity of abiotic stress responses, in which water potential, ionic homeostasis, turgor regulation, and metabolic energy conservation are the central physiological variables[5,6].
Abscisic acid (ABA), often termed the 'stress hormone', is the master coordinator of plant responses to abiotic stress. Its role, however, extends far beyond simple hormonal signaling: ABA functions as a systemic integrator that reprograms cellular metabolism, activates energy conservation programs, modulates the root–shoot communication axis, and establishes epigenetically encoded stress memory[7,8]. Mounting evidence positions ABA not as a passive stress responder but as the molecular anchor of a proposed distinct stable regulatory configuration (herein referred to as the ABA-dominant abiotic stress tolerance state) that the plant's signaling network can adopt in response to osmotic, thermal, or ionic perturbations[9]. We use this term as a conceptual extension of plant immunity frameworks to abiotic contexts, acknowledging that it differs from classical biotic 'immune states'; the terminological basis of this choice is explicitly discussed in the manuscript.
The concept of a hypothetically multistable plant regulatory network, in which the system can occupy discrete, self-sustaining hormonal states, represents a significant departure from linear pathway models[9,10]. Under this framework, the SA-dominant state mediates resistance to biotrophic pathogens, the JA/ET-dominant state governs defense against necrotrophic pathogens and herbivores, the ABA-dominant state coordinates abiotic stress tolerance, and the TOR (target of rapamycin)-dominant growth state supports development and biomass accumulation under favorable conditions[10,11]. Critically, these states do not operate in isolation: Extensive crosstalk, antagonism, and synergy among ABA, SA, JA/ET, and TOR create a dynamically regulated network capable of fine-tuned, context-dependent responses[10]. In addition to these four axes, auxin, cytokinins, brassinosteroids, and gibberellins play well-documented roles in stress adaptation and growth–defense balance, as discussed in the Discussion and Conclusions sections.
The present review addresses existing gaps by (1) delineating the molecular architecture of ABA signaling, including the newly characterized Raf-like MAP kinase kinase kinase (RAF) kinase activation pathway for SnRK2; (2) articulating the concept and mechanistic basis of the ABA-dominant abiotic stress tolerance state; (3) critically examining hormonal crosstalk, metabolic adaptation, reactive oxygen species (ROS)/NO signaling, and autophagy within this state; (4) analyzing the ABA–TOR antagonism as a growth–survival switch, citing the foundational primary research demonstrating the SnRK2–regulatory-associated protein of mTOR (RAPTOR) interaction; (5) evaluating the modulatory roles of nutrients, biostimulants, and the root microbiome; (6) discussing epigenetic mechanisms underpinning stress memory; and (7) identifying the current limitations and future research priorities.
-
ABA biosynthesis is initiated in plastids from the C40 carotenoid zeaxanthin via a series of oxidative cleavage steps. The rate-limiting enzyme 9-cis-epoxycarotenoid dioxygenase (NCED), particularly the NCED3 and NCED9 isoforms, catalyzes the oxidative cleavage of 9-cis-epoxycarotenoids to xanthoxin, which is subsequently converted to ABA in the cytosol by short-chain alcohol dehydrogenase/reductase (ABA2) and the molybdenum-cofactor-dependent abscisic aldehyde oxidase (AAO3)[7,12]. Drought, high temperatures, and osmotic stress rapidly upregulate the transcription of NCED3, establishing a direct coupling between stress perception and hormone biosynthesis. ABA catabolism is mediated primarily by CYP707A cytochrome P450 hydroxylases, providing a counterbalancing attenuation mechanism[12].
An often overlooked dimension of ABA homeostasis is the rapid mobilization of glucose-conjugated reserves (ABA-glucosyl esters [ABA-GEs]) by apoplastic β-glucosidases, which allows a fast surge of active ABA independently of de novo biosynthesis[12]. Intercellular and long-distance ABA transport is mediated by ATP-binding cassette transporters (ABC transporters): ABCG25 exports ABA from biosynthetic cells, whereas ABCG40 facilitates its import into target cells, including guard cells and phloem-loading tissues[13]. The xylem carries ABA primarily as the inactive ABA-GE form, which is hydrolyzed in distal organs, ensuring precise spatiotemporal control of active hormone concentrations.
The PYR/PYL–PP2C–RAF–SnRK2 core signaling module
-
The canonical ABA signaling cascade operates through a three-component perception-derepression-activation mechanism[14,15]. In the absence of ABA, type 2C protein phosphatases (PP2Cs), notably ABI1, ABI2, HAB1, and PP2CA, constitutively dephosphorylate and inactivate sucrose nonfermenting 1-related protein kinases 2 (SnRK2.2, SnRK2.3, and SnRK2.6/open stomata 1 [OST1]), maintaining them in an inactive state. The binding of ABA to pyrabactin resistance (PYR)/PYR1-like (PYL)/regulatory component of ABA receptor (RCAR) receptor proteins promotes the formation of stable ABA–PYL–PP2C ternary complexes, sterically occluding PP2C's active site and thereby releasing SnRK2 kinases from tonic inhibition[14,15].
An important refinement of the SnRK2 activation mechanism that must be incorporated is the role of RAF (Raf-like mitogen-activated protein kinase kinase kinase) kinases. Recent primary research has demonstrated that Group III SnRK2 kinases (SnRK2.2, SnRK2.3, and SnRK2.6) cannot undergo autophosphorylation and self-activation in isolation; instead, B1/B2/B3 RAF kinases phosphorylate SnRK2 in the activation loop, enabling catalytic activation. Furthermore, BIK1 phosphorylates SnRK2 to preferentially engage the PP2C interaction, and PP2C dephosphorylates B2/B3 RAF kinases in their P-loop to sustain basal kinase activity. These mechanistic details, established by primary research, substantially refine the classical PYR/PYL–PP2C–SnRK2 model and should be recognized in any current synthesis of ABA signaling[15].
Liberated SnRK2s subsequently phosphorylate a broad suite of downstream targets: AREB/ABF (ABA-responsive element binding) transcription factors, which activate hundreds of stress-response genes; SLAC1 slows the anion channel, which mediates efflux of Cl− and HCO3− from guard cells; the guard cell outward rectifying K+ channel (GORK) is involved in the outward K+ channel; and respiratory burst oxidase homolog F (RBOHF) nicotinamide adenine dinucleotide phosphate (NADPH) oxidase links ABA signaling to ROS production[15−17]. Stomatal closure integrates ion channel regulation, cytosolic Ca2+ elevation, and ROS signaling into a coherent effector program[16−18]. Recent work has revealed that calcium-dependent protein kinase 15 (CPK15) acts upstream of OST1 in activating SLAC1 under certain conditions, indicating pathway redundancy that buffers the robustness of stomatal closure[19].
Regarding the crosstalk among ABA, TOR, and SnRK2, it has been demonstrated that SnRK2 directly phosphorylates RAPTOR, the scaffold subunit of the TOR Complex 1 (TORC1), thereby establishing a direct molecular link between ABA signaling and TOR inhibition. This finding was subsequently confirmed by independent studies, firmly establishing the SnRK2–RAPTOR interaction as a mechanistically validated regulatory mechanism. In addition, bacterial effectors have been shown to target the SnRK2–ABA signaling pathway, promoting the formation of an apoplastic water film that links ABA-mediated regulation of plant water status with defense against pathogen infection.
Downstream transcriptional regulation
-
AREB/ABF transcription factors recognize the ABA-responsive element (ABRE; PyACGTGGC) in the promoters of stress-responsive genes, including those encoding LEA (late embryogenesis abundant) proteins, dehydrins, osmoprotective enzymes (NCED3, RD29A, RD29B), and antioxidant enzymes[19]. Transcriptomic studies in Arabidopsis thaliana and crop species have identified thousands of ABA-regulated transcripts, underscoring the hormone's role as a master transcriptional switch during stress[8]. In parallel, ABA activates calcium-dependent protein kinases (CPKs) and MAP kinases, which phosphorylate distinct sets of targets and contribute to the specificity and grading of responses[20]. In wheat (Triticum aestivum) and barley (Hordeum vulgare), AREB/ABF homologs control drought-responsive genes, including HVA1 (a LEA protein gene) and DREB1/CBF family members, demonstrating conservation of the transcriptional module in crop species[8].
-
The prevailing PTI/ETI model of plant immunity describes a largely binary pathogen-centric system. However, this model insufficiently captures the full defensive architecture of plants, which must simultaneously manage biotic and abiotic threats in variable environments[3,4]. An alternative systems-level perspective conceptualizes plants' immunity and stress adaptation as a hypothetically multistable network capable of occupying discrete stable regulatory configurations, each defined by the dominance of a particular hormonal axis, such as SA, JA/ET, ABA, or TOR-mediated growth[9]. Each proposed state is maintained by positive feedback loops and bounded by cross-inhibitory interactions with competing states[9,10].
To clarify the terminology, the use of 'immune state' to describe ABA-mediated abiotic stress tolerance requires explicit justification. Classical plant immunity (PTI, ETI, SAR, ISR) is biotic-stress-centered and focuses on the recognition and suppression of pathogens. In the present review, we use 'ABA-dominant state' as a conceptual extension, recognizing that (1) abiotic and biotic stress responses share core signaling nodes (ROS, SnRK1, autophagy, hormonal crosstalk); (2) the ABA-dominant state overlaps functionally with the concept of induced systemic tolerance (IST); and (3) a systems-level view of plant regulatory states necessarily encompasses both biotic and abiotic responses.
We also provide a caveat regarding multistability. Direct empirical evidence for discrete 'attractors' in the mathematical sense, with defined basins of attraction and bifurcation dynamics, remains limited. Most support for multistability is inferred from genetic epistasis studies, hormone antagonism experiments, and transcriptomic clustering analyses rather than from time-resolved dynamic modeling of complete hormone networks[10]. Future work combining synthetic biology approaches with quantitative systems modeling is needed to rigorously test multistability predictions.
Operational definition of the ABA-dominant state
-
We begin this section by explicitly distinguishing the ABA signaling pathway from the ABA-dominant state as a network-level configuration.
The ABA signaling pathway refers to the following molecular cascade: NCED-mediated ABA biosynthesis → PYR/PYL receptor binding → PP2C inhibition → RAF kinase-mediated SnRK2 activation → downstream phosphorylation of SLAC1, AREB/ABF, and RBOHF. This is a molecular mechanism operating at the level of individual cells and tissues. The ABA-dominant state, by contrast, is a proposed system-level regulatory configuration in which the ABA signaling pathway is dominant across the plant signaling network, sustaining its own activity via positive feedback, suppressing competing hormonal states (TOR, SA), and producing a coherent set of organism-level outputs. The key 'attractor' property (if valid) is that the state is self-sustaining and requires active perturbation to exit, rather than simply reflecting transient hormone elevation.
The ABA-dominant abiotic stress tolerance state can be operationally defined by the following co-occurring features: (1) Elevated endogenous ABA concentrations sufficient to saturate high-affinity PYL receptors; (2) active SnRK2.2/2.3/2.6 kinase signaling sustained by RAF kinase activation and PP2C inhibition; (3) suppression of TORC1 activity via SnRK2-mediated phosphorylation of RAPTOR and SnRK1-mediated inhibitory phosphorylation; (4) transcriptional upregulation of ABRE-containing stress genes (RD29A/B, RAB18, LEA, dehydrins); (5) stomatal closure and reduced transpiration; (6) accumulation of compatible solutes (proline, trehalose, raffinose, betaine); and (7) activated autophagy as a cellular recycling platform[7,9,21].
Functionally, the ABA-dominant state parallels IST, a concept proposed to capture the systemic, microbiome-inducible component of abiotic stress tolerance, rather than the biotic-stress-centered SAR and ISR[22]. A critical distinction from classical biotic immunity is the absence of hypersensitive response (HR) or deliberate cell death. Whereas ETI frequently involves the sacrifice of cells at the infection site to limit pathogens' spread, the ABA-dominant state prioritizes the preservation of cellular and tissue integrity through osmoprotection, antioxidant reinforcement, and autophagic homeostasis[3,9]. This represents a fundamentally different regulatory logic: Containment of damage through structural and metabolic fortification rather than through immune-mediated cell sacrifice (Table 1).
Table 1. Comparison of the four proposed regulatory attractor states in the SA–JA/ET–ABA–TOR network.
Feature SA-dominant state JA/ET-dominant state ABA-dominant state TOR-dominant (growth) state Major triggers Biotrophic pathogens, PAMPs, effectors Necrotrophic pathogens, herbivory, wounding Drought, salinity, heat, osmotic stress, low water potential Nutrient repletion, high sucrose/glucose, favorable temperature and light Key hormonal signals ↑SA; ↓AUX, GA, CK ↑JA, ↑ET; ↓GA (DELLA stabilised) ↑ABA; ↓CK, AUX, GA; partial suppression of SA ↑AUX, GA, BR, CK; ↓ABA, SA, JA Core signaling components NPR1, ICS1, TGA factors, PR1 COI1, JAZ, MYC2, ERF1, PDF1.2 NCED3, PYR/PYL, PP2C, SnRK2.6/OST1, AREB/ABF, RAF kinases TOR–RAPTOR–LST8 (TORC1), S6K1/2, eIF4E, BZR1, ARF TOR/SnRK1 status ↓TOR; ↑SnRK1 (moderate) Moderate ↓TOR; partial SnRK1 activation ↓TOR (SnRK2-mediated RAPTOR phosphorylation; SnRK1 co-activation); ↑SnRK1; ↑autophagy ↑TOR; ↓SnRK1; ↑T6P; high ATP/AMP; ↓autophagy Physiological outputs PR gene expression, SAR, growth restriction Phytoalexins, protease inhibitors, ISR, moderate growth inhibition Stomatal closure, osmoprotectant accumulation (proline, trehalose, LEA proteins), ROS/NO signaling; autophagic recycling; epigenetic stress memory Ribosome biogenesis, cell cycle progression, anabolic metabolism, organ expansion Representative marker genes NPR1, ICS1, PR1, TGA2 MYC2, ERF1, PDF1.2, COI1 NCED3, RD29A/B, RAB18, SnRK2.6 (OST1), SLAC1 TOR, S6K1/2, CYCD, BZR1, ARF -
The interactions among plant hormones combine antagonism, synergy, and context-dependence that is rarely captured by simple linear models[10,23]. The relationship between ABA and SA exemplifies this complexity. In many contexts, ABA suppresses SA-mediated defenses: Elevated ABA attenuates the function of NPR1 (Nonexpresser of PR Genes 1) function, reduces the expression of ICS1 (isochorismate synthase 1), and promotes the degradation of SA signaling intermediates, thereby dampening SAR during abiotic stress when resources must be redirected from energetically expensive immune activation[23,24]. Conversely, SA can partially inhibit ABA signaling by stabilizing PP2C phosphatases, highlighting reciprocal suppression as a mechanism of hormonal competition[24] (Fig. 1).
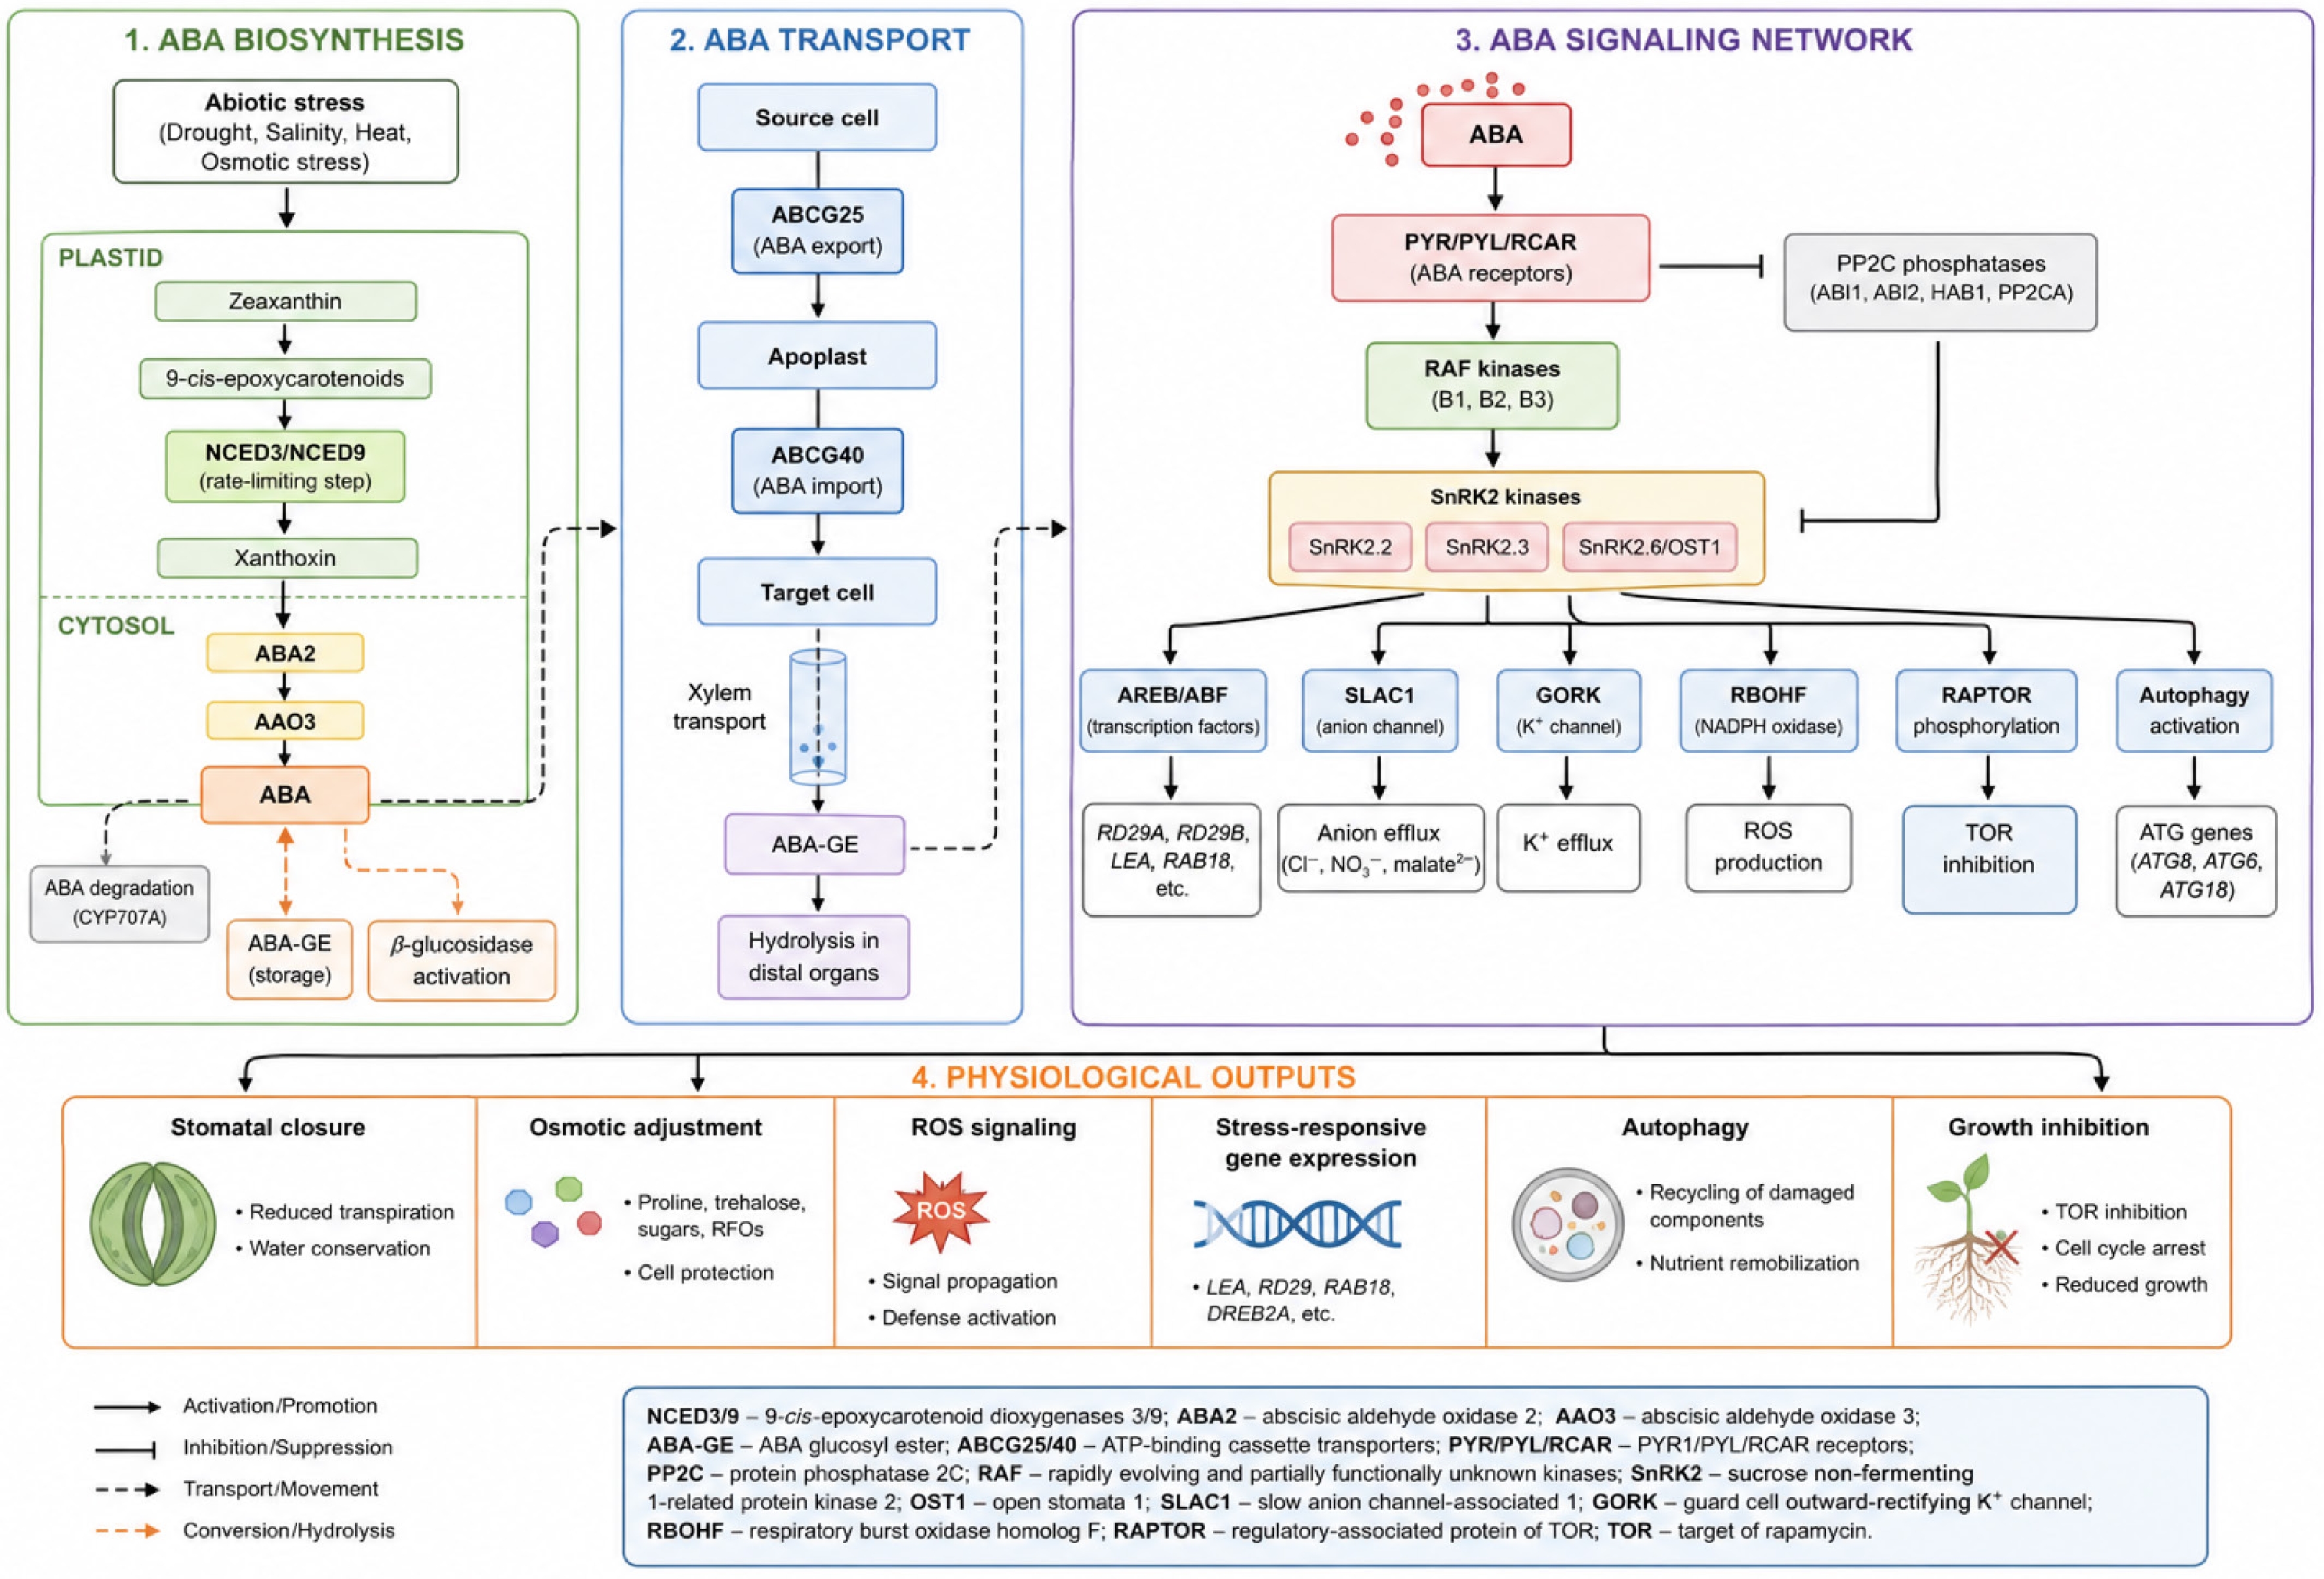
Figure 1.
Integrated network of ABA biosynthesis, transport, signaling, and downstream physiological responses. (1) Abiotic stress perception induces ABA biosynthesis through the plastidial carotenoid pathway involving NCED3/NCED9, ABA2, and AAO3. (2) ABA homeostasis is regulated by CYP707A-mediated catabolism, ABA-GE hydrolysis by β-glucosidases, and ABA transport via ABCG25/ABCG40 transporters. (3) Perception of ABA by PYR/PYL/RCAR receptors inhibits PP2C phosphatases, enabling RAF–SnRK2 kinase activation and downstream phosphorylation events. (4) Activated SnRK2 coordinates physiological adaptation through regulation of AREB/ABF, SLAC1, GORK, RBOHF, and RAPTOR, integrating ABA signaling with stomatal closure, osmotic adjustment, ROS signaling, autophagy activation, and growth inhibition.
The ABA–JA/ET relationship is more nuanced. JA and ABA share several signaling nodes—notably ROS-mediated activation of MAP kinase cascades, SnRK1 activation, and autophagic induction—creating the potential for synergistic cooperation under combined biotic–abiotic stress[23,25]. Indeed, drought-stressed plants frequently show altered susceptibility to necrotrophic pathogens, likely reflecting ABA–JA/ET cross-modulation[25]. However, ABA can also suppress JA-induced protease inhibitor expression under conditions where water conservation is prioritized, illustrating that synergy is conditional and concentration-dependent[23]. A landmark study demonstrated that bacterial effectors can target the SnRK2 pathway to create a water apoplast during infection, directly linking ABA-mediated water regulation to biotic stress contexts and illustrating that the boundaries between ABA-dominant and biotic immune states are flexible.
The ABA–TOR axis constitutes perhaps the most functionally consequential hormonal interaction in the context of abiotic stress. TOR kinase, which integrates nutrient, light, and energy signals to drive anabolic growth, is negatively regulated by SnRK1, the central energy sensor activated by ABA signaling[26,27]. Crucially, SnRK2 kinases directly phosphorylate RAPTOR, a TORC1 scaffold subunit, inhibiting TOR activity. This is distinct from SnRK1-mediated RAPTOR phosphorylation and provides a direct molecular bridge from ABA perception to TOR suppression. Conversely, active TOR phosphorylates SnRK1 and ABA signaling components, suppressing the stress response during favorable conditions[27]. This reciprocal antagonism establishes a proposed bistable molecular switch controlling the growth–survival trade-off, discussed in detail in the Conclusions section.
Growth-promoting hormones, such as auxin, cytokinin, brassinosteroids (BRs), and gibberellins (GAs), play important roles in the regulatory network that deserve explicit discussion beyond the SA–JA/ET–ABA–TOR core. Auxins such as indole-3-acetic acid (IAA) suppress SA-dependent defenses and partially antagonize ABA-mediated growth inhibition through auxin response factor (ARF)-dependent gene expression; during recovery from abiotic stress, rising auxin levels promote meristematic re-activation and cell elongation. Cytokinins (CK) antagonize ABA responses: CK levels rise in shoots during recovery, promoting stomatal opening and stimulating TOR signaling, thereby accelerating the transition from ABA-dominant to TOR-dominant states. Brassinosteroids activate TOR via the BRI1–BSK1 pathway and suppress SA/JA signaling, positioning them as growth-dominance promoters; yet at low concentrations, BR can enhance basal stress tolerance. Gibberellins inactivate DELLA repressors that otherwise restrict growth and can partially suppress ABA responses through phytochrome-interacting factor (PIF) activity[27]. The integration of these growth-promoting hormones adds further regulatory flexibility, allowing the plant to calibrate its balance among immunity, stress tolerance, and growth.
-
Stomatal closure represents the most rapid and ecologically direct consequence of ABA elevation, occurring within minutes of hormone perception. Guard cell ABA signaling integrates Ca2+ signals generated by OSCA/HCO3−-sensitive channels, ROS produced by RBOHD/F, and K+/anion channel regulation[16,28]. OST1/SnRK2.6 phosphorylates SLAC1 at multiple serine residues, activating anion efflux; GORK channels simultaneously mediate K+ efflux; and the combined loss of osmolytes collapses guard cell turgor[16,29]. Recent primary research has demonstrated that OST1 activates SLAC1 primarily through CPK15, revealing a regulatory hierarchy within ABA–stomatal signaling that differs from earlier models and highlights CPK15 as a key integrator[29]. Aquaporins of the plasma membrane intrinsic protein (PIP) and tonoplast intrinsic protein (TIP) families are regulated by ABA through transcriptional downregulation and post-translational phosphorylation, reducing membranes' water conductivity and limiting transpirational water loss[8].
In crop species, ABA-mediated stomatal control has been extensively characterized. In maize (Zea mays), guard cell ABA signaling follows a similar PYR/PYL–PP2C–SnRK2 logic but with expanded PYL receptor families. In wheat, ABA-induced stomatal closure provides critical drought tolerance under field conditions. Including these crop-relevant examples strengthens the translational applicability of the framework.
Osmolyte accumulation and structural protection
-
Under the ABA-dominant state, carbon flux is redirected from growth-supporting biosynthesis toward the accumulation of compatible solutes. Proline synthesis, governed by the P5CS1 and P5CS2 enzymes, is strongly ABA-induced and provides osmotic adjustment, protein stabilization, ROS scavenging, and signaling functions[30]. Trehalose accumulation stabilizes proteins and membranes and, through the signaling metabolite trehalose-6-phosphate (T6P), modulates the SnRK1–TOR balance[31]. Raffinose family oligosaccharides (RFOs) provide both cryoprotection and antioxidant activity[30].
LEA proteins and dehydrins, which are intrinsically disordered proteins that accumulate during late embryogenesis and stress, form a molecular shield around cellular structures, preventing aggregation and membrane collapse during dehydration[19]. Their induction is directly controlled by ABF/AREB transcription factors via ABRE elements. Cell wall remodeling reinforces structural integrity under osmotic stress and limits uncontrolled water movement[9,32]. In soybean (Glycine max) and rice (Oryza sativa), the accumulation of ABA-inducible LEA proteins under drought has been documented in primary research, demonstrating the relevance of these osmoprotective mechanisms to crops[8].
Carbon−nitrogen balance and metabolic reprogramming
-
The ABA-dominant state involves a fundamental shift in carbon−nitrogen (C/N) metabolism. SnRK1, activated by energy deprivation and ABA, phosphorylates and inhibits key anabolic enzymes, including nitrate reductase, sucrose phosphate synthase, and ADP-glucose pyrophosphorylase, while concurrently activating catabolic enzymes and sugar-mobilizing genes[26]. The resulting increase in the C/N ratio favors osmoprotectant synthesis and limits nitrogen-expensive processes such as ribosome biogenesis and cell cycle progression[26,32]. Nitrogen's availability, through its influence on SnRK1 activity and TOR signaling via nitrogenous metabolite sensing, therefore functions as a critical modulator of the intensity of the ABA response[33].
-
Reactive oxygen species (ROS) play a paradoxical dual role in ABA signaling, acting as both secondary messengers that are essential for signal propagation and as potentially cytotoxic molecules requiring stringent detoxification[17,34]. ABA rapidly stimulates the production of superoxide radicals (O2·−) through RBOHD and RBOHF NADPH oxidases, directly activated by SnRK2 kinases and calcium-dependent protein kinases[17]. Dismutation of O2·− by superoxide dismutase (SOD) yields H2O2, a more stable and membrane-permeable molecule that serves as the primary ROS signaling messenger[34]. H2O2 activates Ca2+-permeable channels in the plasma membrane and directly oxidizes cysteine residues in key regulatory proteins[17,34].
During early ABA signaling, catalase (CAT) activity is transiently suppressed, allowing ROS to accumulate to signaling concentrations[35]. Subsequently, antioxidant systems are progressively induced: Ascorbate peroxidase (APX) detoxifies H2O2 in the chloroplasts and the cytosol; glutathione reductase (GR) regenerates reduced glutathione (GSH); and the ascorbate–glutathione cycle ensures sustained removal of H2O2[34,35]. A particularly important phenomenon is the intercellular 'ROS wave', mediated by sequential activation of respiratory burst oxidase homolog (RBOH) proteins in adjacent cells, which propagates stress signals across tissues at speeds of several centimeters per minute, coordinating systemic responses beyond the primary stress site[34].
Nitric oxide as a co-regulator of ABA responses
-
Nitric oxide (NO) functions in close coordination with ROS within ABA signaling. ABA promotes NO synthesis primarily via nitrate reductase (NR)-mediated reduction of nitrite, and NO acts synergistically with H2O2 to promote stomatal closure[36,37]. The primary biochemical mechanism is S-nitrosylation (the reversible addition of an NO group to cysteine thiols), which modifies the activity of key regulators including SnRK2.6/OST1, RBOHD, APX, and GAPDH[36]. S-nitrosylation of RBOHD by NO can limit ROS production, establishing a negative feedback mechanism that prevents excessive oxidative bursts[37]. The stable S-nitrosoglutathione (GSNO) formed from NO and GSH serves as a reservoir and long-range NO carrier, contributing to systemic NO signaling. NO also inhibits components of the TOR complex via S-nitrosylation, reinforcing the transition from growth to survival mode[36].
Autophagy as a stress survival platform
-
Autophagy has emerged as a central regulatory platform in the ABA-dominant state, extending far beyond its originally characterized role in nutrient recycling under starvation[38,39]. ABA promotes autophagy through multiple converging mechanisms: SnRK1 phosphorylates and inhibits TORC1, relieving TOR-mediated suppression of the ATG1/ATG13 autophagy initiation complex; SnRK2-mediated RAPTOR phosphorylation provides an additional direct route from ABA signaling to TOR suppression and activation of autophagy; and ABA-regulated transcription factors upregulate the expression of ATG8, ATG6, and ATG18[38,39].
Autophagy under ABA dominance serves several distinct functions: (1) Degradation of oxidatively damaged proteins and organelles, (2) selective chloroplast autophagy (chlorophagy), (3) recycling of cytoplasmic nitrogen and carbon to support osmoprotectant synthesis, and (4) modulation of ABA signaling itself, through selective autophagic degradation of PP2C phosphatases, creating a positive feedback loop that sustains the ABA-dominant state[38,39].
-
TOR is a conserved serine/threonine kinase that acts as the central integrator of nutrient, energy, and hormonal signals to drive anabolic growth[27,40]. In TORC1, the primary TOR complex in plants, TOR associates with RAPTOR and LST8 to phosphorylate S6K1/2 kinases and eIF4E-binding proteins, thereby stimulating ribosome biogenesis, mRNA translation, and cell growth[27]. Under favorable conditions, TOR suppresses SnRK1 by direct phosphorylation of its catalytic subunit, maintaining a high-growth state.
Under abiotic stress, elevated ABA activates SnRK2 kinases. Primary research first demonstrated that SnRK2 directly phosphorylates RAPTOR, thereby directly linking ABA signaling to TOR inhibition independently of SnRK1. In parallel, SnRK1 (activated by falling adenosine triphosphate/adenosine monophosphate [ATP/AMP] ratios) also phosphorylates multiple TORC1 components[26,27]. Together, these two convergent phosphorylation events, i.e., SnRK2→RAPTOR and SnRK1→TORC1, drive TOR into an inactive state and establish the proposed bistable switch between growth and survival states[27,40]. The transition from the TOR-dominant to the ABA-dominant state entails a comprehensive metabolic shift: Protein synthesis drops sharply as ribosomes are inactivated, cell cycle progression is arrested at the G1/S checkpoint, and photosynthetic carbon assimilation decreases through stomatal closure and reduced Calvin cycle-related enzyme activity[27,40].
Additionally, bacterial effectors target the SnRK2–ABA signaling pathway to generate an apoplastic water film that facilitates bacterial colonization. This finding positions the SnRK2 pathway at the intersection of abiotic and biotic stress responses, adding a biotic stress dimension to the concept of the ABA-dominant state.
Post-stress reactivation of TOR and growth recovery
-
The re-establishment of TOR dominance upon relief from stress is equally well-orchestrated. Recovery of sucrose levels and nitrogen availability activates TOR through Ras-related guanosine triphosphatase (RAG)-like complexes, resuming ribosome biogenesis, meristematic activity, and organelle proliferation[27,40]. BRs and GAs facilitate the reactivation of TOR and partially antagonize ABA signaling during recovery. Cytokinins (CKs), rising in shoots as root stress is relieved, promote stomatal opening and stimulate TOR signaling, contributing to the ABA → TOR transition. Nitrogen deficiency increases SnRK1 activity, shifting the balance toward ABA dominance and promoting resource conservation[33]. Phosphorus availability influences TOR via its effect on ATP concentrations[41] (Fig. 2).
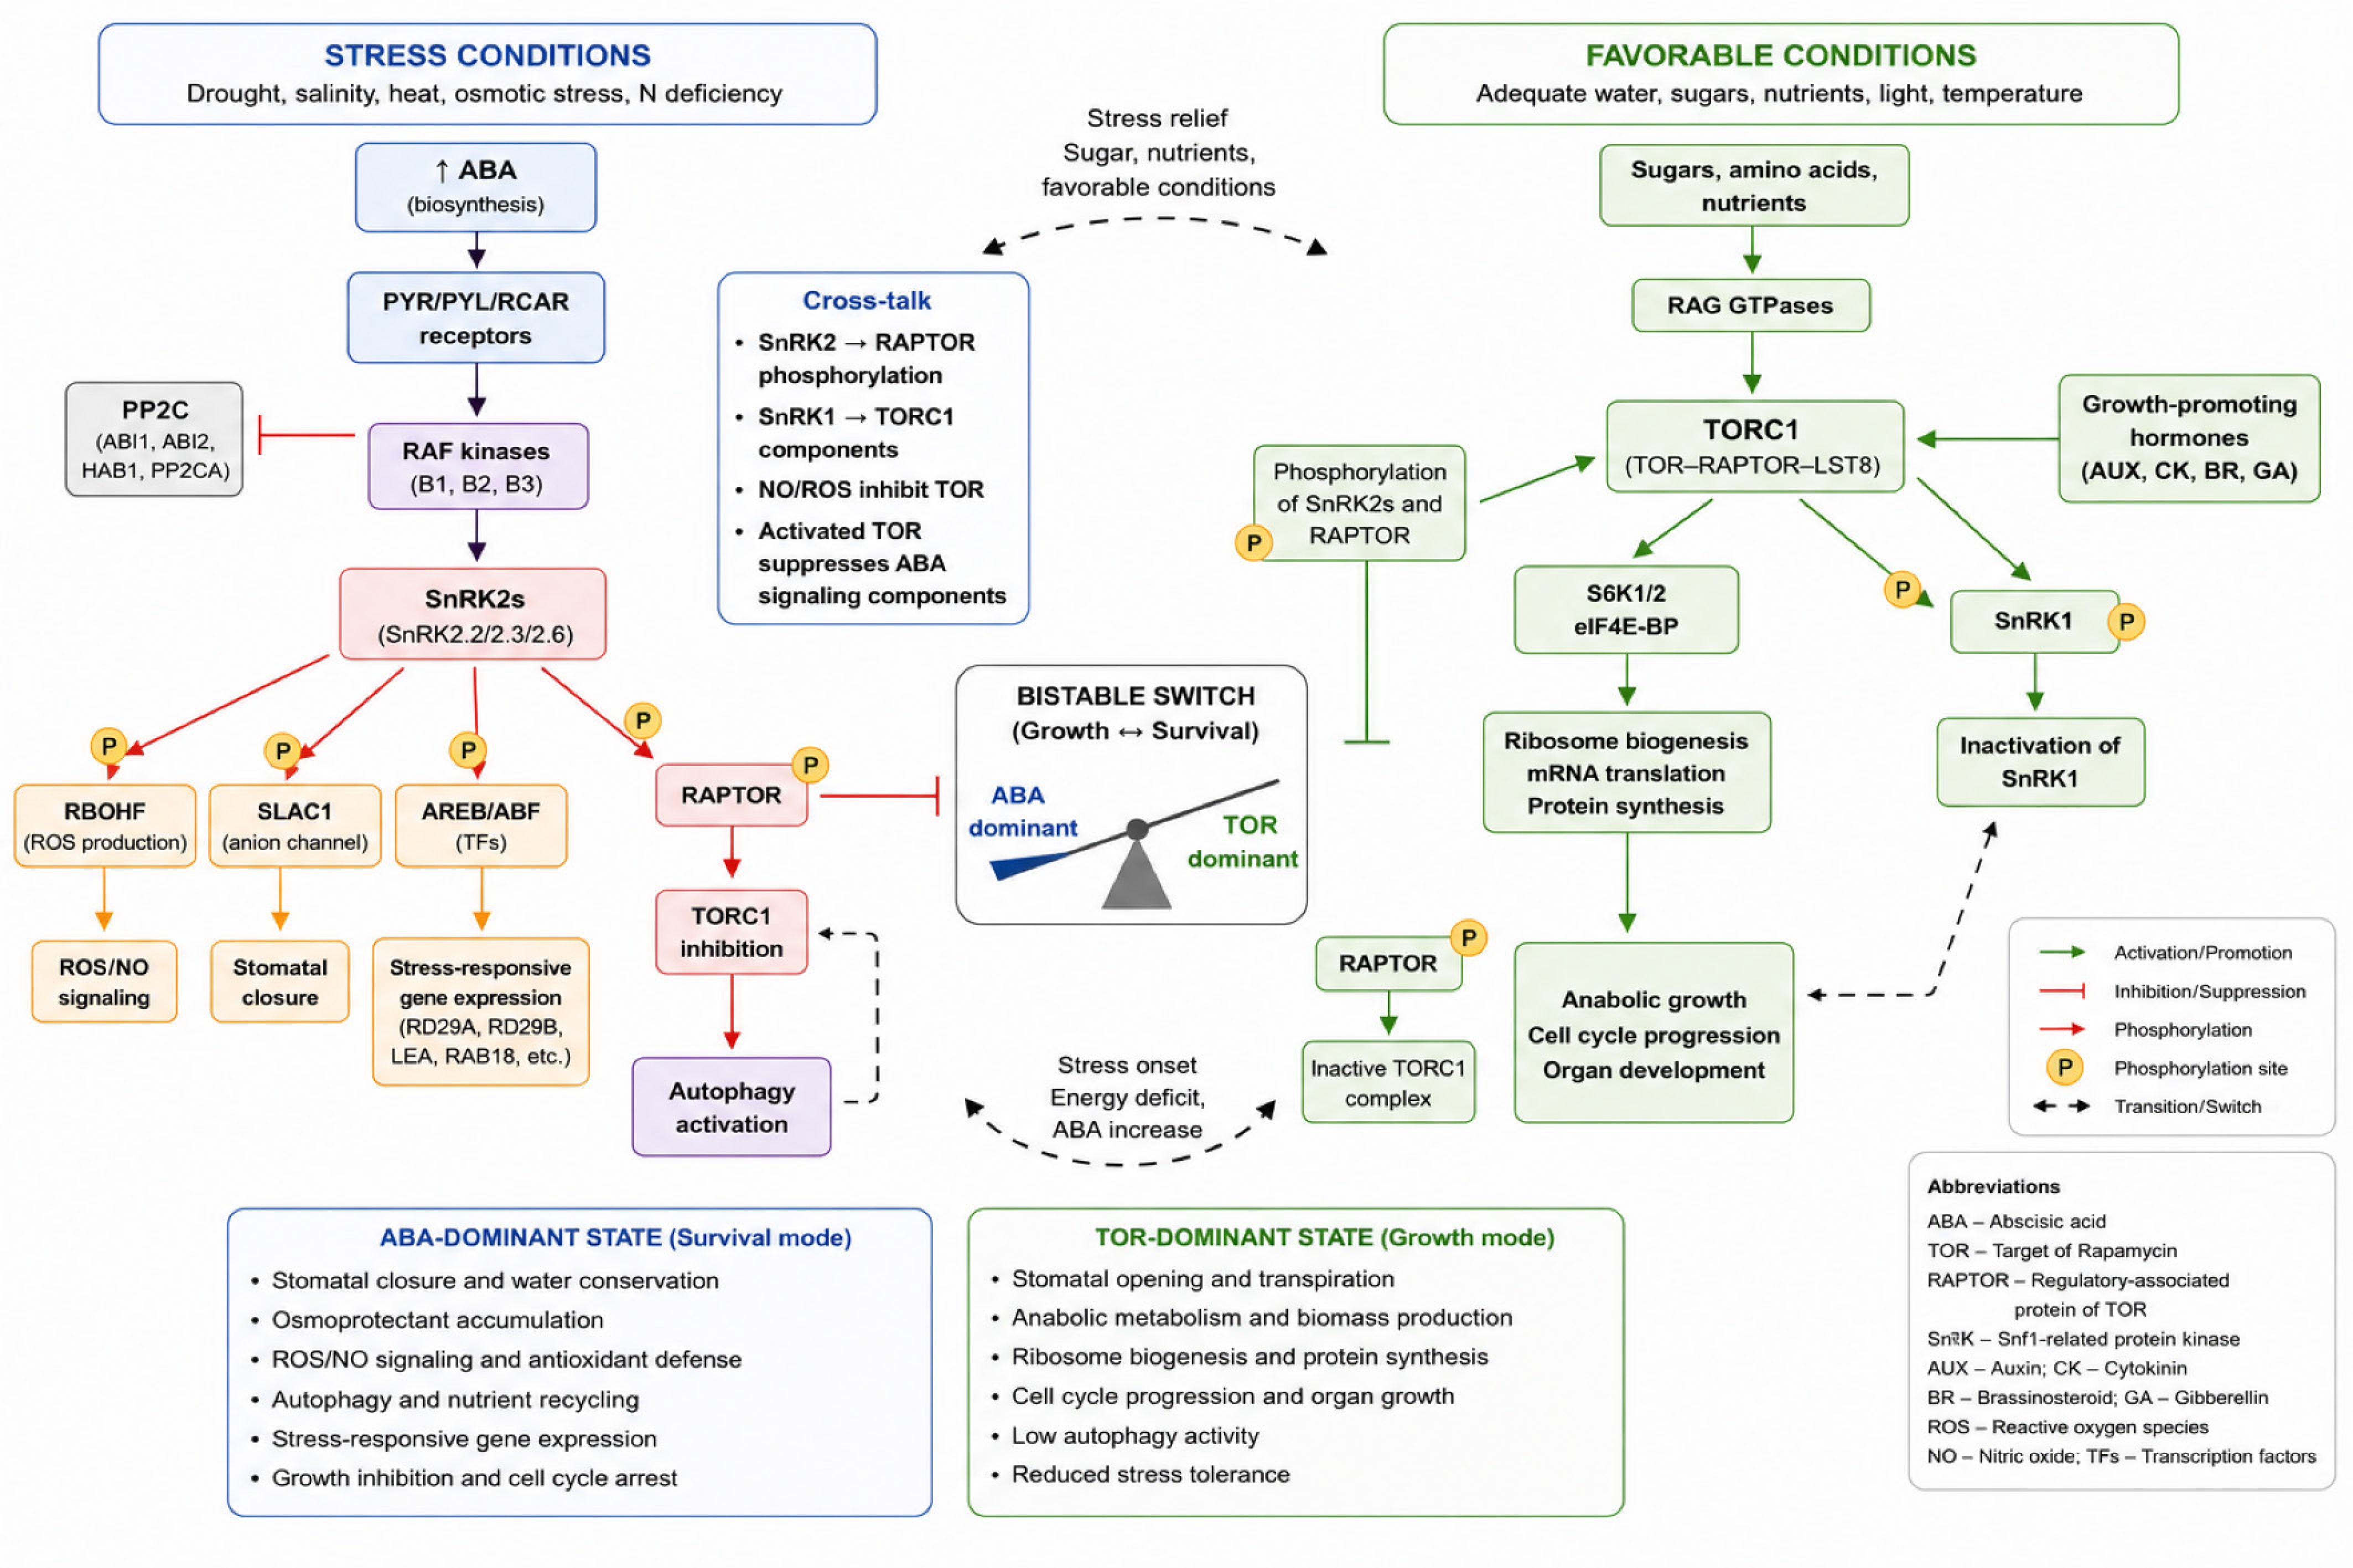
Figure 2.
Proposed ABA–TOR bistable molecular switch controlling the transition between stress survival and growth. Under abiotic stress, ABA signaling activates the PYR/PYL–PP2C–RAF–SnRK2 cascade, resulting in phosphorylation of RAPTOR, suppression of TORC1 activity, activation of autophagy, and induction of stress-adaptive responses. Under favorable conditions, TOR signaling promotes anabolic metabolism, ribosome biogenesis, protein synthesis, cell cycle progression, and organ growth while repressing ABA-mediated stress responses. The reciprocal antagonism between ABA and TOR represents a proposed bistable regulatory switch coordinating plant adaptation to changing environmental conditions.
-
Mineral nutrients are not merely structural components of cellular biochemistry but are also active modulators of ABA-dependent signaling. Potassium (K+) plays a particularly direct role: K+ efflux from guard cells through GORK channels is essential for ABA-induced stomatal closure, and adequate K+ nutrition ensures the electrochemical capacity for rapid stomatal responses[29,42]. Calcium (Ca2+) is indispensable as a secondary messenger in ABA signaling: ABA-stimulated Ca2+ influx activates CPKs and calcium-dependent protein kinase (CDPK) cascades that phosphorylate SLAC1 and SnRK2.6, amplifying both stomatal and transcriptional responses[20,28].
Micronutrients play essential roles in antioxidant defense. Manganese and copper are cofactors for Mn-SOD and Cu/Zn-SOD, respectively, thereby reducing O2·− accumulation[43]. Zinc is required for Cu/Zn-SOD activity. Sulfur is the elemental backbone of GSH, and sulfur deficiency significantly compromises cellular antioxidant capacity[43]. Molybdenum, as a cofactor of nitrate reductase, influences the NO/ABA balance[37].
Osmoprotectants and organic biostimulants
-
Exogenous application of compatible solutes can prime ABA-mediated responses. Proline application reduces the ABA accumulation needed for osmotic adjustment while maintaining membranes and enzymes[30]. Trehalose modulates the SnRK1–TOR balance via trehalose-6-phosphate (T6P) signaling, and exogenous application of trehalose has been shown to enhance drought and heat tolerance in multiple crop species[31]. Polyamines (spermidine, spermine, putrescine) stabilize membrane architecture, activate autophagy, and modulate ROS homeostasis in coordination with ABA[44]. Melatonin reduces ABA-induced ROS toxicity and promotes autophagy at appropriate concentrations[44].
Seaweed extracts, particularly those derived from Ascophyllum nodosum and other brown algae, moderate ABA responses without blocking stress adaptation mechanisms[45]. Microbial biostimulants, such as plant growth-promoting rhizobacteria (PGPR) and their exopolysaccharides, enhance ABA signaling in roots and prime SnRK2-dependent responses, while phosphites activate ABA-mediated autophagic programs[46,47].
-
The root microbiome has emerged as a critical regulator of plant hormonal networks, with direct implications for the ABA-dominant abiotic stress tolerance state[22,47]. PGPR, particularly Bacillus subtilis, Pseudomonas fluorescens, and Paenibacillus polymyxa, can enhance ABA signaling in roots by activating the expression of NCED3/NCED9, thereby accelerating stomatal closure and osmoprotective responses to water deficit[48]. However, the magnitude and direction of PGPR's effects on ABA signaling are highly dependent on the plant species, microbial strain, soil conditions, and stress intensity. For example, effects observed in tomato (Solanum lycopersicum) or A. thaliana may differ substantially from those in wheat or maize under field conditions. Generalizations from model systems to crops therefore require empirical validation.
PGPR-based modulation of ABA is context-dependent and bidirectional: Many PGPR attenuate ABA levels in leaves while maintaining root ABA signaling[47,49]. Bacterial exopolysaccharides further contribute by forming a hydrogel-like matrix around root surfaces, physically reducing soil water desorption stress[50].
Arbuscular mycorrhizal fungi: systemic ABA modulators
-
Arbuscular mycorrhizal fungi (AMF), particularly Rhizophagus irregularis, establish obligate symbioses with the roots of most terrestrial plant species and substantially alter ABA-dependent stress physiology[51,52]. AMF improve phosphorus, magnesium, and micronutrient uptake, directly reducing the need for elevated ABA to mobilize stored mineral reserves under stress. Similar to PGPR's effects, AMF–ABA interactions are strain-specific and depend on the plant species; the outcomes reported for specific AMF strains in wheat or maize may not extrapolate to other crop–fungal combinations. AMF also modulate ABA signaling through ROS homeostasis: Mycorrhizal roots maintain lower basal H2O2 levels and show higher SOD and APX activities[52]. Furthermore, AMF activate JA-dependent pathways in roots, interacting with ABA to enhance cross-tolerance to drought, salinity, and pathogens simultaneously[51,52].
Endophytes, actinomycetes, and integrated microbiome function
-
Endophytic bacteria and fungi residing within plant tissues fine-tune ABA signaling from within, producing moderate ROS levels that prime SnRK2 without triggering toxic oxidative phases, and supplying IAA and CKs that moderate ABA accumulation while preserving growth capacity[53]. Actinomycetes, particularly Streptomyces spp., activate NCED3 in roots and produce signaling molecules that promote early formation of stress memory[54]. Again, these effects are reported for specific strain–plant combinations and should not be overgeneralized; the species and environmental context are critical determinants of the outcomes.
The integrated picture reveals a complex microbiome–ABA–plant axis in which different microbial guilds contribute complementary regulatory functions[47−54] (Fig. 3).
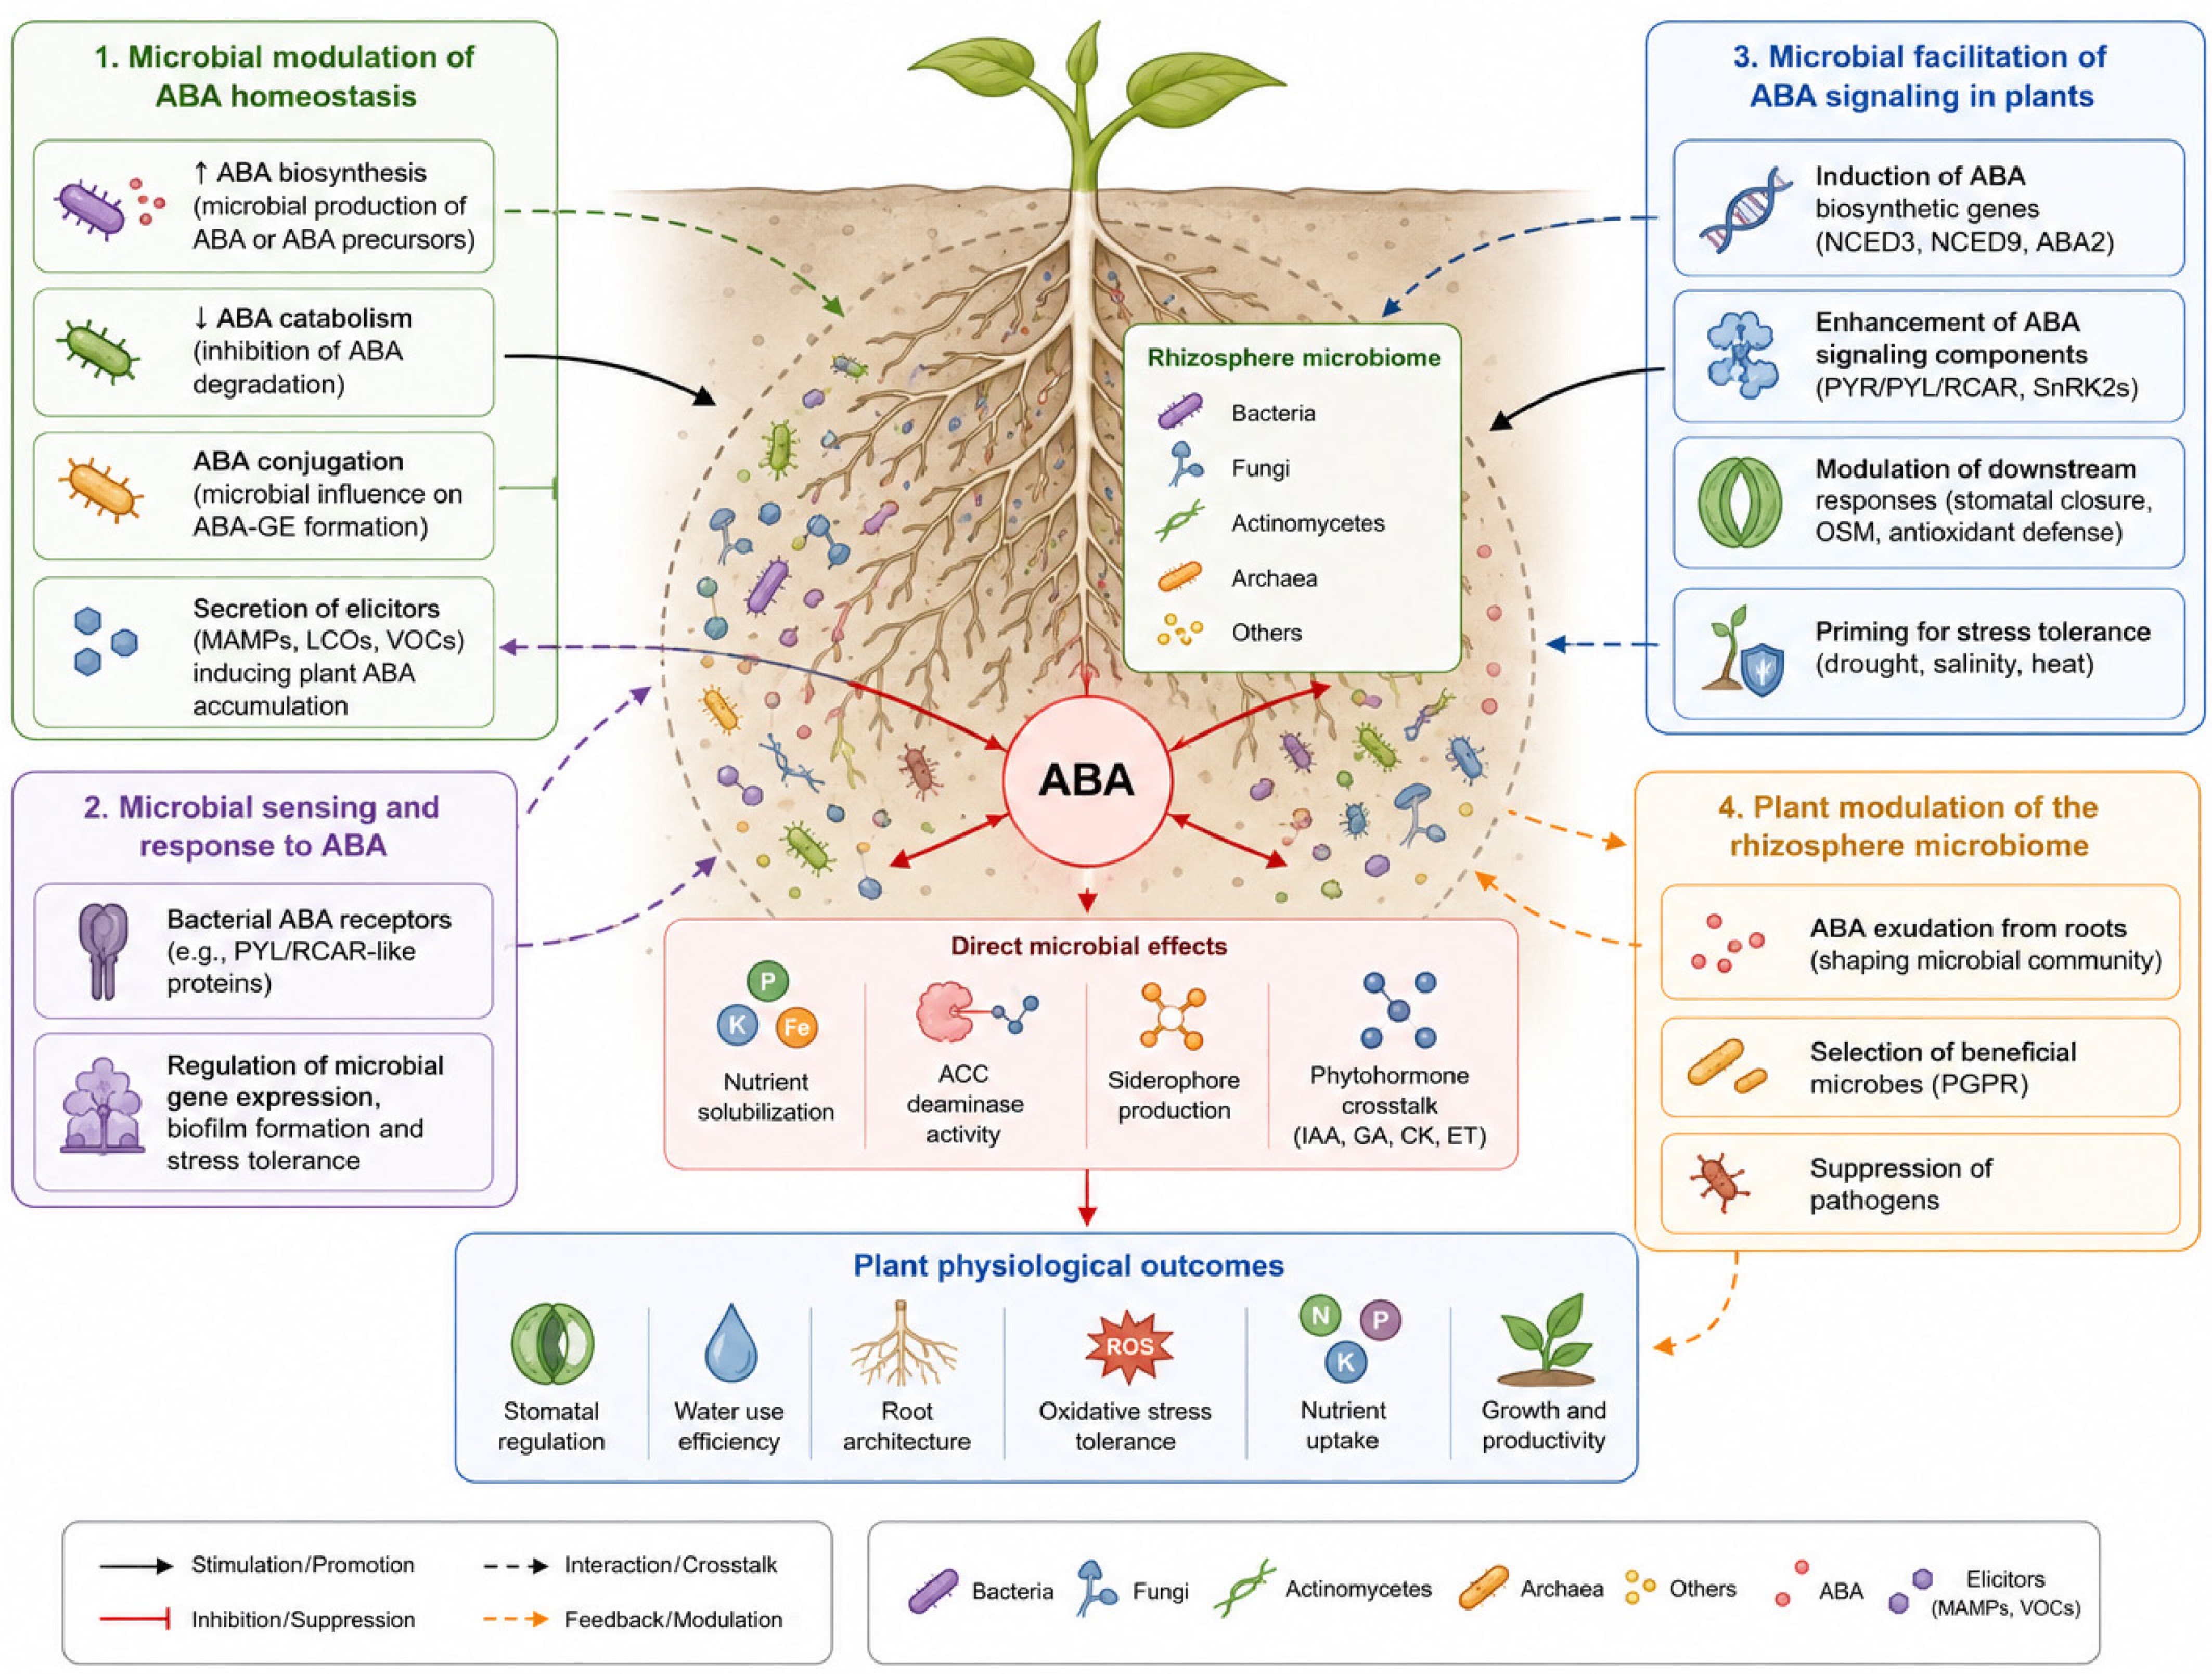
Figure 3.
Integrated microbiome–ABA interaction network in the rhizosphere. The rhizosphere microbiome functions as an integrated regulatory system that modulates the ABA-dominant abiotic stress tolerance state. PGPR, AMF, endophytes, and actinomycetes regulate ABA biosynthesis (NCED3), PYR/PYL–PP2C–RAF–SnRK2 signaling, ROS homeostasis, nutrient acquisition, and phytohormone balance. These complementary microbial activities promote osmoprotection, autophagy, stress-responsive gene expression, and epigenetic stress memory, thereby enhancing plants' adaptation and resilience under abiotic stress.
-
The ABA-dominant response extends beyond short-term physiological changes to encompass long-term restructuring of gene expression mediated by epigenetic modifications and noncoding RNAs[7,8]. ABA promotes increased methylation of the promoters of growth-related genes (TOR, expansins), suppressing growth programs, while simultaneously facilitating the demethylation of stress-adaptive genes (RD29A, NCED3, DREB2A) through the activity of ROS1 and DEMETER (DME) demethylases[8].
Dynamic chromatin remodeling occurs via histone modifications: H3K4me3, an activating mark, accumulates on stress-adaptive genes under ABA signaling; H3K27me3, a repressive mark within the Polycomb PRC2 complex, is removed from stress-responsive genes; and H3K9ac activates transcription of ABA-regulated genes[7]. Key ABA-regulated noncoding RNAs include miR159 (represses MYB33/MYB101), miR398 (regulates CSD1/CSD2 expression), and siRNAs that mediate the RNA-directed DNA methylation (RdDM) pathway[8]. Epigenetic 'memory marks' such as H3K4me3 on stress-responsive genes (RD29B, HSPs, LEA) can persist for weeks after water balance is restored, priming the transcriptional machinery for rapid reactivation[8]. In crop species, stress memory via H3K4me3 has been documented in maize and barley, supporting the translational relevance of these mechanisms[8].
-
The ABA-dominant abiotic stress tolerance state concept presented here constitutes a meaningful extension of classical plant immunity frameworks rather than a replacement of them. PTI and ETI remain robust descriptors of the recognition of and response to pathogens, and SAR and ISR adequately capture the systemic dimensions of biotic immunity[3,4]. The innovation of the hypothetically multistable network model is to position these pathogen-oriented states alongside the ABA-dominant and TOR-dominant states as equipotent configurations of the same underlying regulatory machinery[9,10].
A particularly important conceptual contribution is the recognition that the ABA-dominant state is not simply an 'off switch' for biotic immunity but an active, energy-optimized, self-sustaining regulatory configuration with its own effector programs, memory mechanisms, and systemic propagation routes[9,22]. The terminological use of 'immune state' for ABA-mediated abiotic tolerance is an intentional conceptual extension, not a claim of identity with biotic immunity. Under simultaneous or rapidly alternating stresses (e.g., drought + heat + pathogens), the plant regulatory network likely occupies intermediate or hybrid configurations that are not adequately described by any single attractor state. The model should be understood as a conceptual framework that is applicable under defined conditions rather than a universal description of all plant states[55−67]. Tissue-specific, developmental-stage-dependent, and species-specific differences in state transitions also require recognition.
Biotechnological and agricultural implications
-
The framework of the ABA-dominant abiotic stress tolerance state has direct implications for crop improvement. Genetic enhancement of ABA signaling components, such as NCED3, PYL receptors with increased ABA affinity, or SnRK2.6 with enhanced stability, offers routes to constitutively or conditionally enhanced stress tolerance[7,8]. Engineering or identifying crop variants with optimized RAF kinase activity could provide enhanced SnRK2 activation without the metabolic costs of elevated ABA concentrations.
Biostimulant design can be rationalized using the ABA signaling cascade as a template: Compounds that enhance early ABA biosynthesis (beta-glucosidase inducers), stabilize SnRK2 activity, or prime autophagy (spermidine, phosphites) could be combined in formulations that engage multiple regulatory nodes for synergistic stress protection[44−46]. Microbiome engineering to design inoculant consortia that provide complementary ABA-modulatory functions represents a systemic approach to stress tolerance[47,53,68−71].
-
The ABA-dominant abiotic stress tolerance state emerges from this synthesis as a conceptually cohesive and mechanistically rich regulatory configuration occupying a central place in the plant hormonal network. It is defined by coordinated ABA biosynthesis and signaling, RAF kinase-mediated and PP2C-gated SnRK2 activation, and SnRK2-mediated RAPTOR phosphorylation, as well as SnRK1-mediated TOR inhibition, ROS/NO secondary messaging, autophagic cellular recycling, osmoprotectant accumulation, and epigenetically encoded stress memory. As one of four proposed interacting regulatory configurations in a hypothetically multistable network alongside SA-, JA/ET-, and TOR-dominant states, it enables plants to mobilize a comprehensive, energetically optimized survival strategy under abiotic challenge.
Future research should prioritize (1) quantitative systems biology approaches, including mathematical modeling of hormone networks' dynamics, to rigorously test the hypothetical multistability hypothesis and map the state transition parameters; (2) single-cell and spatially resolved transcriptomics to map the cell-type specificity of components of the ABA-dominant state; (3) field-based studies using multiple stress combinations (drought + heat + pathogens) to test whether the multistable network model predicts the observed immune–stress response hierarchies in crop species; (4) systematic characterization of the recently elucidated RAF kinase module in diverse crop species; (5) engineering of microbiome consortia with defined, complementary ABA-modulatory functions; and (6) rigorous evaluation of epigenetic ABA memory for crop improvement applications. The ABA-dominant abiotic stress tolerance state represents a central platform for climate resilience, linking molecular plant biology with sustainable agricultural innovation.
This research did not receive any specific grant from funding agencies in the public, commercial, or not-for-profit sectors.
-
During the preparation of this work, the authors used NotebookLM and Claude (Anthropic) (Version/date: 2025–2026) for language refinement, grammar checking, and style editing. The authors reviewed and edited all content, verified its accuracy, and take full responsibility for the integrity and originality of the final manuscript. No AI tool is credited as an author.
-
The authors confirm their contributions to the paper as follows: study conception and design: Khablak SH, Bondareva LM; literature analysis and critical evaluation: Khablak SH, Bondareva LM, Abdullaieva YA, Spychak VM; writing – original draft, scientific supervision: Khablak SH; writing – review and editing: Abdullaieva YA, Kolomiiets YV. All authors reviewed the results and approved the final version of the manuscript.
-
Data sharing is not applicable to this article as no datasets were generated or analyzed during the current study.
-
The authors declare that they have no conflict of interest.
- Copyright: © 2026 by the author(s). Published by Maximum Academic Press on behalf of Chongqing University. This article is an open access article distributed under Creative Commons Attribution License (CC BY 4.0), visit https://creativecommons.org/licenses/by/4.0/.
-
About this article
Cite this article
Khablak SH, Bondareva LM, Kolomiiets YV, Abdullaieva YA, Spychak VM. 2026. The ABA-dominant abiotic stress tolerance state: an integrative framework for abscisic acid-mediated abiotic stress tolerance in plants. Plant Hormones 2: e023 doi: 10.48130/ph-0026-0021 

The ABA-dominant abiotic stress tolerance state: an integrative framework for abscisic acid-mediated abiotic stress tolerance in plants
- Received: 21 April 2026
- Revised: 13 July 2026
- Accepted: 05 August 2026
- Published online: 10 September 2026
Abstract: Abscisic acid (ABA) is a pivotal phytohormone orchestrating plants' adaptations to abiotic stresses, yet its role as a distinct homeostatic regulatory state within the broader plant hormonal signaling network remains conceptually underexplored. Classical models of plant immunity—centered on pattern-triggered immunity (PTI) and effector-triggered immunity (ETI)—do not fully account for the systemic, energy-optimizing responses that plants deploy against drought, salinity, extreme temperatures, and osmotic stress. Here, we present a critical synthesis of current evidence supporting the concept of an ABA-dominant abiotic stress tolerance state as one of four interacting proposed stable regulatory configurations within a hypothetically multistable metabolic signaling network, salicylic acid (SA)–jasmonate and ethylene (JA/ET)–ABA–target of rapamycin (TOR). We clarify that this designation represents a metaphorical extension of immune terminology to encompass coordinated abiotic stress regulatory states, and acknowledge that direct mathematical evidence for attractor-level multistability remains limited. We analyze the molecular architecture of ABA signaling, encompassing 9-cis-epoxycarotenoid dioxygenase-mediated biosynthesis, pyrabactin resistance (PYR)/PYR1-like (PYL)/regulatory component of ABA receptor (RCAR) receptor activation, Raf-like MAP kinase kinase kinase (RAF) kinase-mediated SnRK2 activation, Type 2C protein phosphatase (PP2C) inhibition, and downstream SnRK2 kinase cascades that coordinate stomatal closure, osmoprotectant synthesis, reactive oxygen species (ROS)/NO homeostasis, and autophagic recycling. We further examine the antagonistic interplay between ABA and the TOR kinase complex as a central growth–survival switch, emphasizing the critical role of SnRK2-mediated regulatory-associated protein of mTOR (RAPTOR) phosphorylation as established in primary research. Epigenetic mechanisms—including histone modifications, DNA methylation, and noncoding RNA networks—are considered as substrates for ABA-dependent stress memory and cross-generational tolerance. The ABA-dominant abiotic stress tolerance state represents a mechanistically coherent and biotechnologically relevant platform for engineering climate-resilient crop plants.